Introduction
In response to the development and spread of herbicide-resistant weeds, the agricultural industry has commercialized new weed control systems on the basis of use of crop cultivars with genetically modified resistance to auxin herbicides (Behrens et al. Reference Behrens, Mutlu, Chakraborty, Dumitru, Jiang, LaVallee, Herman, Clemente and Weeks2007; Egan et al. Reference Egan, Barlow and Mortensen2014; Feng and Brinker Reference Feng and Brinker2014; Mortensen et al. Reference Mortensen, Egan, Maxwell, Ryan and Smith2012; Richburg et al. Reference Richburg, Wright, Braxton and Robinson2012; Wright et al. Reference Wright, Shan, Walsh, Lira, Cui, Song, Zhuang, Arnold, Lin, Yau, Russell, Cicchillo, Peterson, Simpson, Zhou, Ponsamuel and Zhang2010). Corteva Agriscience’s (Dow AgroSciences, 9330 Zionsville Road, Indianapolis, IN 46268) Enlist™ Weed Control System is based on the use of cotton, soybean [Glycine max (L.) Merr.], and corn (Zea mays L.) cultivars with genetically modified resistance to 2,4-D, glyphosate, and glufosinate (Richburg et al. Reference Richburg, Wright, Braxton and Robinson2012; Wright et al. Reference Wright, Shan, Walsh, Lira, Cui, Song, Zhuang, Arnold, Lin, Yau, Russell, Cicchillo, Peterson, Simpson, Zhou, Ponsamuel and Zhang2010). Enlist™ cotton cultivars express resistance to 2,4-D conferred by a transgene encoding an aryloxyalkanoate dioxygenase that metabolizes 2,4-D to an herbicidally inactive form (Richburg et al. Reference Richburg, Wright, Braxton and Robinson2012). 2,4-D has long been used for selective control of broadleaf weeds in monocots, including turfgrass, cereal, and pastures (Pokorny Reference Pokorny1941). Widespread adoption of Enlist™ cotton may occur in the future due to the efficacy of 2,4-D in controlling dicot weeds and the relatively low incidence of 2,4-D–resistant weed species (Heap Reference Heap2018). Furthermore, the history of off-target auxin herbicide movement onto susceptible crops may motivate producers to adopt a defensive strategy by planting auxin-resistant cultivars (Egan et al. Reference Egan, Barlow and Mortensen2014; Mortensen et al. Reference Mortensen, Egan, Maxwell, Ryan and Smith2012).
Although Enlist™ cotton cultivars express resistance to 2,4-D, other cultivars susceptible to 2,4-D are still commonly used. Cotton susceptibility to 2,4-D damage has been reported consistently since the commercialization of 2,4-D (Marple et al. Reference Marple, Al-Khatib, Shoup, Peterson and Claassen2007, Reference Marple, Al-Khatib and Peterson2008; Staten Reference Staten1946). The number of off-target deposition events involving auxin herbicides has reached 2,708 total complaints of dicamba damage to more than 1.4 million ha of soybean during 2017 (Bradley Reference Bradley2017). Herbicide drift, spray equipment contamination, spraying during temperature inversions, and the use of formulations with a propensity for volatilization compound the risk associated with adoption of the auxin technologies (Egan et al. Reference Egan, Barlow and Mortensen2014; Mortensen et al. Reference Mortensen, Egan, Maxwell, Ryan and Smith2012). Off-target deposition can arise from many factors, including auxin herbicide persisting in spray equipment such as spray tanks, hoses, and nozzles (Boerboom Reference Boerboom2004; Cundiff et al. Reference Cundiff, Reynolds, Thomas and Mueller2017).
Noticeable symptoms on susceptible crops exposed to auxin herbicides cause auxin herbicide injury to be frequently reported in agriculture (Egan et al. Reference Egan, Barlow and Mortensen2014). Leaf malformation, stem and petiole epinasty, and necrosis on susceptible species all may follow exposure to 2,4-D (Marple et al. Reference Marple, Al-Khatib, Shoup, Peterson and Claassen2007; Sciumbato et al. Reference Sciumbato, Chandler, Senseman, Bovey and Smith2004). Johnson et al. (Reference Johnson, Fisher, Jordan, Edmisten, Stewart and York2012) concluded that cotton lint yield was reduced as a result of exposure to 2,4-D amine rates of 269, 78, 20, 5, and 1 g ai ha−1 on 20- to 30-cm cotton. Everitt and Keeling (Reference Everitt and Keeling2009) evaluated non–2,4-D tolerant cotton response to 2,4-D rates of 280, 28, 2.8, and 0.28 g ai ha−1 and found that 28 g ai ha−1 reduced lint yield by up to 50% if exposure occurred from the cotyledon to five-leaf growth stage and by 68% at the pinhead square stage. Egan et al. (Reference Egan, Barlow and Mortensen2014) found that cotton at late vegetative and early squaring stages is most susceptible to injury from low rates of 2,4-D. Byrd et al. (Reference Byrd, Collins, Culpepper, Dodds, Edmisten, Wright, Morgan, Baumann, Dotray, Manuchehri, Jones, Grey, Webster, Davis, Whitaker, Roberts, Snider and Porter2015) reported reduced cotton yield following exposure to 2 g 2,4-D ae ha−1 when exposure occurred at growth stages between four-leaf to 2 weeks after full bloom, and further concluded that exposure at any growth stage to 40 g 2,4-D ae ha−1 resulted in yield loss. Overall, the greatest yield impacts were observed from exposure between nine-leaf to 2 wk after full bloom (Byrd 2015).
2,4-D herbicide use and incidences of deposition on susceptible cotton will likely increase in future growing seasons. An experiment was conducted to characterize cotton response to a sublethal concentration of 2,4-D as a function of growth stage at the time of exposure. The objective of this experiment was to determine the cotton growth stages most susceptible to injury and yield loss, and to illustrate any varying effects on yield partitioning as a function of growth stage at exposure.
Materials and method
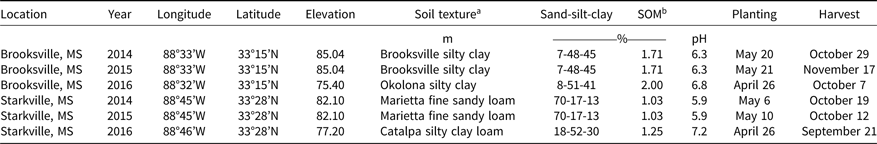
Field studies were conducted during the 2014, 2015, and 2016 growing seasons to characterize cotton sensitivity to a dilute concentration of 2,4-D at several growth stages. Field research was conducted at the R. R. Foil Plant Research Facility in Starkville, MS, and the Black Belt Branch Experiment Station in Brooksville, MS, for a total of 6 site-years of field research; site details are provided in Table 1. The cultivar ‘DP 1321 B2RF’ (Monsanto Company, 800 North Lindbergh Blvd., St. Louis, MO 63167) was seeded at a rate of 128,440 seeds ha−1 and a 2.5-cm depth each year at both locations. It is important to note that this variety is an early-mid maturing cultivar and other cultivars in different maturity groups may respond differently to 2,4-D stress. Experiment plants at each location were in-furrow irrigated and managed with standard production practices recommended by Mississippi State University Extension Service (Anonymous 2018a). Planting was timed such that a high probability of precipitation (>60%) within 24 hours was present, thus ensuring proper germination and crop establishment.
Details of locations of experiments in 2014, 2015, and 2016.

a U.S. Department of Agriculture (2016).
b Abbreviation: SOM, soil organic matter.
Plots consisted of four 97-cm rows, each 12.2 m long, and each experiment was structured as a randomized complete block design. Treatments were different application timings of 2,4-D herbicide (Weedar 64®, Nufarm Americas Inc., 4020 Aerial Center Parkway, Suite 101, Morrisville, NC 27560). The choline salt formulation of 2,4-D is the only formulation approved for use in 2,4-D–resistant crops; however, there is no difference in the response of 2,4-D–sensitive cotton to either amine or choline formulations (Byrd et al. Reference Byrd, Collins, Culpepper, Dodds, Edmisten, Wright, Morgan, Baumann, Dotray, Manuchehri, Jones, Grey, Webster, Davis, Whitaker, Roberts, Snider and Porter2015).
The first application timing occurred PRE immediately after planting, with the subsequent 15 applications being made weekly to separate plots until 14 weeks after emergence (WAE). In a previous study conducted at Mississippi State University, researchers found that a concentration of 8.3 g ae ha−1 is suitable for simulating a sublethal concentration of 2,4-D while also inducing visible injury on susceptible cotton (unpublished data). This concentration fits within the range of those used in previous studies to simulate particle drift or tank contamination rates (Byrd et al. Reference Byrd, Collins, Culpepper, Dodds, Edmisten, Wright, Morgan, Baumann, Dotray, Manuchehri, Jones, Grey, Webster, Davis, Whitaker, Roberts, Snider and Porter2015; Egan et al. Reference Egan, Barlow and Mortensen2014; Johnson et al. Reference Johnson, Fisher, Jordan, Edmisten, Stewart and York2012). Thus, 8.3 g ae ha−1 2,4-D was applied at 4.8 kph using a CO2-pressurized plot backpack sprayer calibrated to deliver 140 L ha−1 at 276 kPa and a four-nozzle spray boom equipped with TTI11002 (TeeJet Technologies, Glendale Heights, IL 60139) spray tips at an elevation of 51 cm above the crop canopy. All applications were made to the center two rows of each plot at a time of low winds (3–8 kph), with the outer row on either side serving as a buffer between plots. No 2,4-D movement between plots was observed at any point during the experiment.
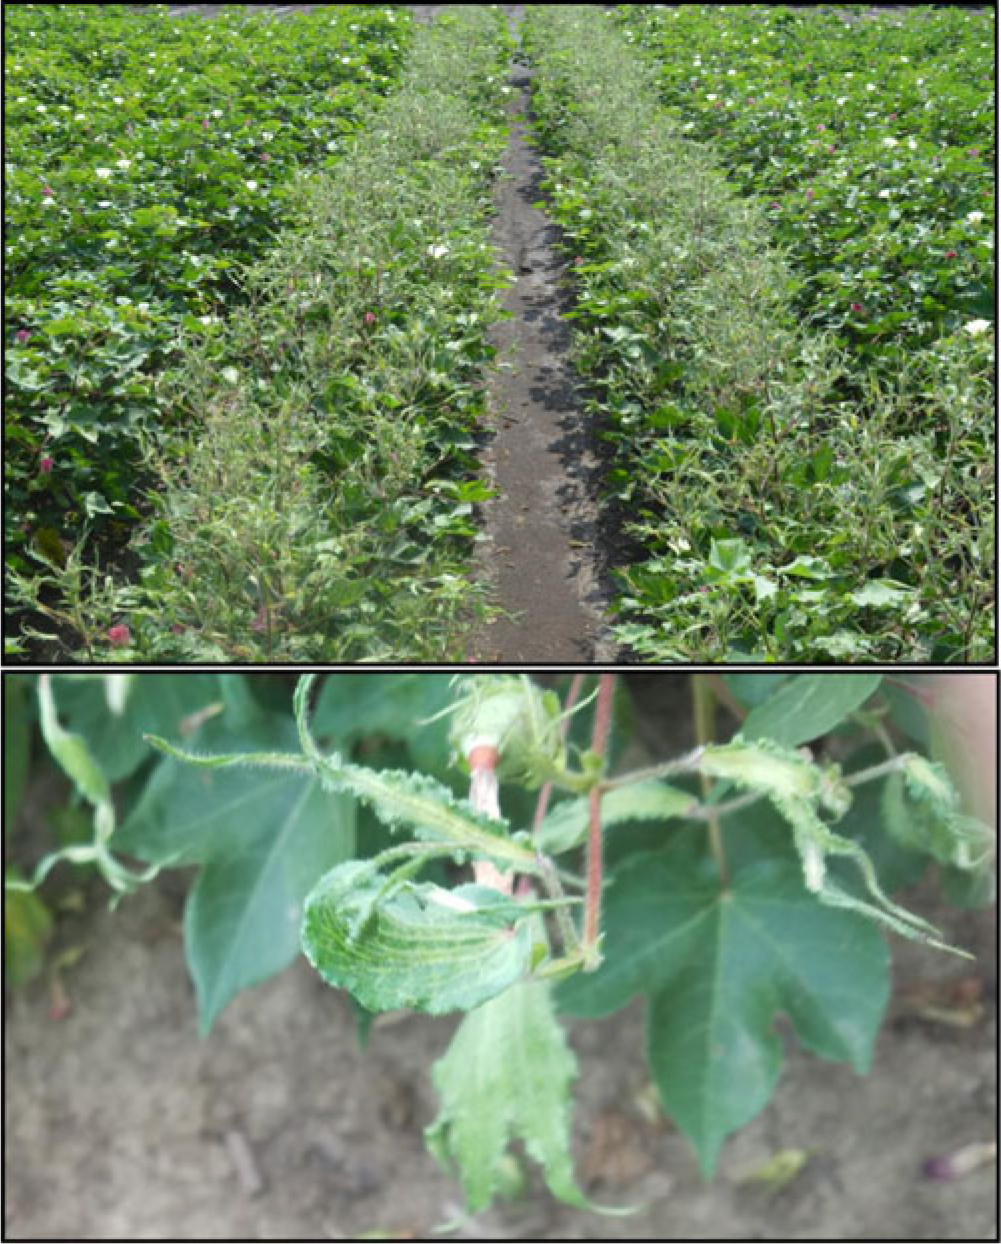
Crop injury evaluations were made throughout the season at intervals of 7, 14, 21, and 28 days after each treatment. Visual injury was evaluated using a 0 to 100 scale (0 = no injury; 100 = complete plant mortality) (Frans et al. Reference Frans, Talbert, Marx, Crowley and Camper1986). The visible symptoms of particular interest in injury evaluation were leaf curling and strapping (Figure 1), petiole and stem epinasty, and changes in crop height. Relative maturity data were evaluated by counting the nodes above cracked boll (NACB) from the center two rows of each plot (Kerby et al. Reference Kerby, Supak, Banks, Snipes, Herber and Richter1992). NACB data were recorded when the nontreated control (NTC) reached boll cutout or when the average number of nodes above white flower for six randomly selected plants in the NTC plots was five or fewer, at approximately 15 to 16 WAE (Bourland et al. Reference Bourland, Oosterhuis and Tugwell1992).
Characteristic cotton injury symptomology from exposure to a dilute concentration of 2,4-D. (Top) Leaf strapping and internode elongation. (Bottom) Close-up of leaf strapping.

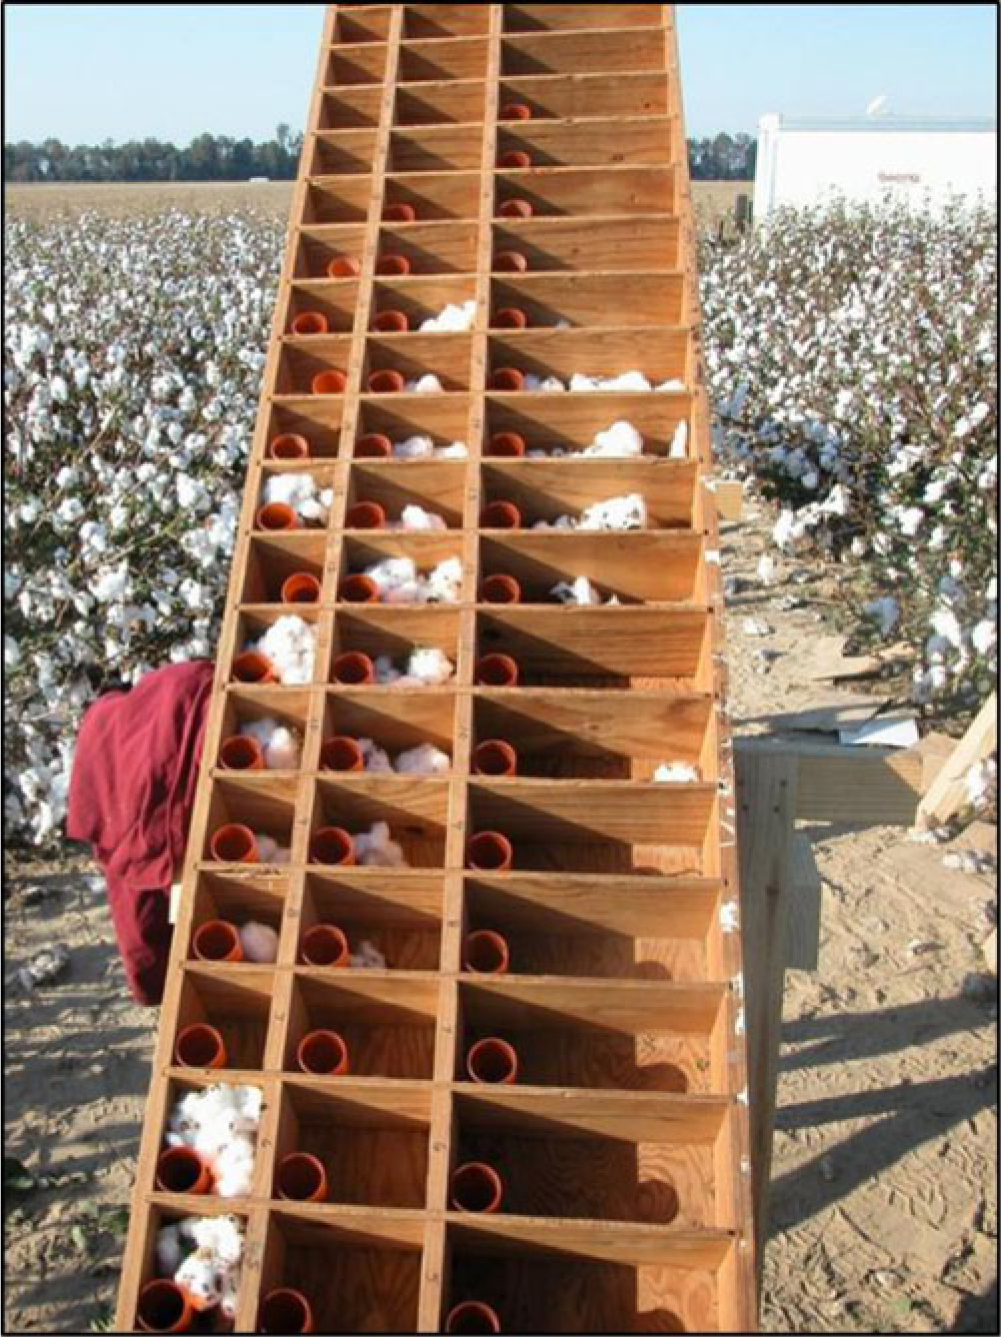
Cotton height was recorded at the time of harvest-aid application from three randomly selected plants in the second and third rows of each plot (six plants total per plot). After defoliation, a 3-m section of plants from the second row of each plot was removed by cutting at the soil surface for plant mapping determinations, using a box partitioned into sections corresponding to fruiting site and nodal position, as shown in Figure 2 (Jenkins et al. Reference Jenkins, McCarty and Parrot1990). Plots were harvested using a two-row plot picker, and machine-harvested seed cotton weight from each plot was determined. In the 2016 experiments, gin turnout data were recorded from a 250-g sample collected from the hand-harvested yield of each plot. Fiber quality was characterized using a high-volume instrument at Texas Tech Fiber and Biopolymer Research Institute (1001 East Loop 289, Lubbock TX 79403).
Box used for partitioning hand-harvested seed cotton used for plant-mapping analyses. Bolls were removed from each plant by fruiting site and partitioned in the corresponding slot on the box.

Machine-harvested seed cotton yield data are presented as percent reductions relative to the NTC yield. Visible crop injury, relative maturity, crop height, and machine-harvested yield reduction data were subjected to ANOVA using the PROC MIXED feature of SAS, version 9.4 (SAS Institute Inc., Cary, NC). Treatment means were separated by Fisher protected LSD at the α = 0.05 level of significance, using the PDMIX800 macro (Saxton Reference Saxton1998). To assess the relationship between exposure timing and cotton response, machine-harvested yield reduction data were regressed by application timing using the PROC REG feature.
Hand-harvested data were subjected to ANOVA and means separation using the PROC MIXED feature of SAS, version 9.4 with Fisher’s protected LSD at the α = 0.05 level of significance. Hand-harvested yield data were analyzed by horizontal position, vertical zone, and maturity cohort. Yield-partitioning data are presented as raw seed cotton weight by position and zone and as a percentage of the total seed cotton weight from each treatment by position and zone. Position 1 consisted of all bolls found in the first fruiting position immediately adjacent to the main stem on each branch, position 2 consisted of all bolls in the next horizontal position, and position 3 consisted of any bolls beyond the second position. Yield was also partitioned vertically into zones. Zone 1 consisted of all bolls taken from sympodial (reproductive) branches up to the eighth main stem node, zone 2 consisted of all bolls taken from sympodial branches on the ninth through 12th nodes, and zone 3 consisted of bolls taken from any sympodial branch beyond node 12 (Huff et al. Reference Huff, Dodds, Irby and Reynolds2010; Jenkins et al. Reference Jenkins, McCarty and Parrot1990). Any bolls harvested from a fruiting site on a monopodial (vegetative) branch were classified as vegetative, and any bolls harvested from any fruiting site on a plant that had lost apical dominance were classified as aborted. Vegetative and aborted classifications were treated as discrete fruiting sites independent of vertical or horizontal partitioning. As such, there are two methods to calculate the sum of the total hand-harvested yield from a given exposure timing: (1) adding the weights corresponding to each position plus the vegetative and aborted weights, or (2) adding the weights corresponding to each vertical zone plus vegetative and aborted weights. Each of these methods should result in the same value.
On the basis of the assumption that cotton exhibits a 6-day horizontal fruiting interval and a 3-day vertical fruiting interval, an analysis was conducted on the basis of fruiting-site maturity cohorts, which contain fruiting structures of the same age. In this system, cohort 5 would contain fruiting structures on node 9 position 1, node 7 position 2, and node 5 position 3 (Huff et al. Reference Huff, Dodds, Irby and Reynolds2010; Jenkins et al. Reference Jenkins, McCarty and Parrot1990). Bednarz and Nichols (Reference Bednarz and Nichols2005) found different values for vertical and horizontal fruiting intervals, ostensibly due to differing environments and varieties. However, the values reported by Jenkins et al. (Reference Jenkins, McCarty and Parrot1990) were used because they were reported for environments similar to those in this experiment.
Year and location were combined as environment during analyses. All data met proper parameter distribution assumptions and any data points with corresponding studentized residual values >2.5 were removed as outliers. Application timing was analyzed as a fixed factor, whereas environment was considered a random factor. In this experiment, we used multiple-environment trials designed to evaluate treatment effects over a broad inference space. Accordingly, data for all parameters (i.e., injury, maturity, height, machine-harvested yield, hand-harvested yield) are presented as treatment means pooled over environment and means for all parameters were separated with Fisher protected LSD (Blouin et al. Reference Blouin, Webster and Bond2011; Carmer et al. Reference Carmer, Nyquist and Walker1989). The use of multiple-environment trials is advantageous in making inferences over a broad range of environmental parameters such as time and space (Blouin et al. Reference Blouin, Webster and Bond2011; Carmer et al. Reference Carmer, Nyquist and Walker1989; Walker et al. Reference Walker, Bond, Ottis, Gerard and Harrell2008; Yang Reference Yang2010).
Results and discussion
Cotton morphological response
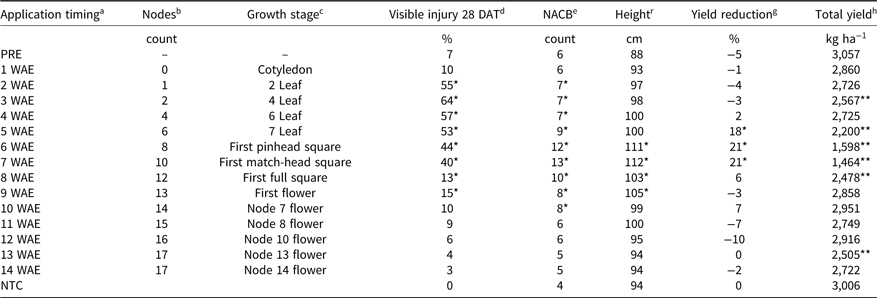
2,4-D causes distinct crop injury in susceptible cotton cultivars that generally is manifested as leaf strapping and stem and petiole epinasty. Loss of apical dominance may occur, usually from exposure at vegetative growth stages. Leaf chlorosis and plant death may ensue, depending on rate (Johnson et al. Reference Johnson, Fisher, Jordan, Edmisten, Stewart and York2012; Marple et al. Reference Marple, Al-Khatib and Peterson2008). Visible evaluations of these crop injury symptoms are often used in estimating the severity of exposure to 2,4-D (Marple et al. Reference Marple, Al-Khatib and Peterson2008; Sciumbato et al. Reference Sciumbato, Chandler, Senseman, Bovey and Smith2004). In these experiments, the most commonly observed crop responses were leaf strapping (Figure 1) and height increases. Data for cotton growth stage at time of exposure, visible crop injury, NACB, crop height, percent machine-harvested yield reduction, and total hand-harvested yield weight by exposure timing pooled over environment are displayed in Table 2. Seasonal (April to November) temperatures were within historical ranges in each experiment and, along with timely in-furrow irrigation, helped ensure that cotton growth stage was similar in all experiments at a given exposure timing.
The effect of application timing on cotton injury, relative maturity, height, yield, and yield reduction as affected by application timing of 2,4-D at 8.3 g ae ha−1 averaged over environment.

a Number of WAE at which application occurred.
b Number of nodes on cotton plants at the time of application.
c At the time of application.
d Abbreviations: DAT, days after each treatment; NACB, nodes above cracked boll; NTC, nontreated check; WAE, weeks after emergence.
e Recorded approximately 15 to 16 WAE.
f Average crop height at defoliation.
g Average machine-harvested seed cotton yield reduction relative to the NTC.
h Total weight of the hand-harvested seed cotton.
* Significantly increased relative to the NTC.
** Significantly decreased relative to the NTC.
Up to 64% cotton injury resulted from exposure to 2,4-D at 2 to 9 WAE. These exposures corresponded to cotton growth stages ranging from two-leaf to beginning bloom, and the effects were consistent with previous findings (Egan et al. Reference Egan, Barlow and Mortensen2014). No significant injury (i.e., 3%–10%) was observed when exposures occurred after 9 WAE (first bloom). Cotton height was increased after 2,4-D exposure 6 to 9 WAE, which corresponded to squaring and early blooming cotton (Table 2). The increase in height from exposure to 2,4-D at these timings was coincident with abortion of early reproductive structures and the consequent reversion to vegetative growth. Delayed maturity in the form of greater NACB counts was observed when exposure to 2,4-D occurred from 2 to 10 WAE on cotton ranging from the two-leaf to mid-bloom stages of growth (Table 2). Delayed maturity can pose a problem in the event of loss-of-heat unit accumulation at the end of the growing season, such as in the event of an early frost, which may result in lost yield potential. 2,4-D exposure 5 to 7 WAE on cotton at late vegetative or early squaring growth stages led to reductions in machine-harvested seed cotton yield of 18% to 21%. Total hand-harvested seed cotton weight was reduced after 2,4-D exposure 3, 5 to 8, or 13 WAE on cotton ranging from vegetative to early reproductive growth stages (Table 2). These results are consistent with previous findings that 2,4-D exposure at late vegetative and early reproductive growth stages leads to reductions in cotton yield (Everitt and Keeling Reference Everitt and Keeling2009; Johnson et al. Reference Johnson, Fisher, Jordan, Edmisten, Stewart and York2012). Polynomial modeling of machine-harvested yield reductions by exposure timing found no adequate models (data not shown).
Hand-harvested and mapped yield data
By horizontal position
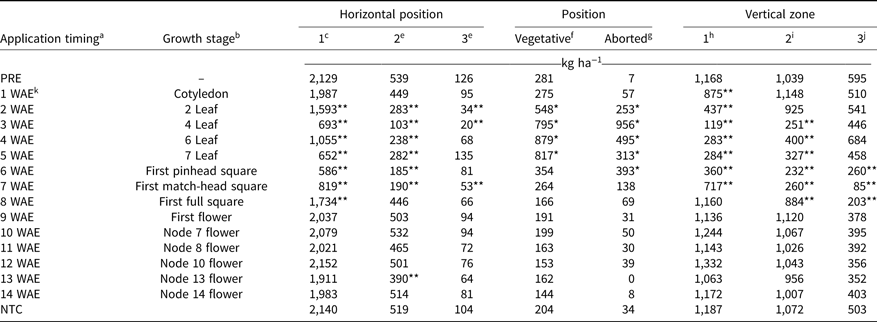
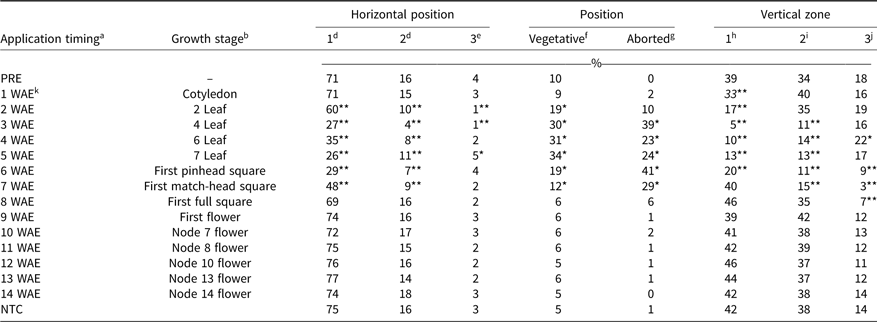
Table 3 lists seed cotton weight by horizontal fruiting position and vertical zone as affected by application timing pooled over environment. Seed cotton weight partitioned in position 1 was reduced from exposure 2 to 8 WAE on cotton ranging from early vegetative to early squaring growth stages. Exposure 2 to 7 or 13 WAE reduced yield partitioned in position 2, and exposure 2, 3, or 7 WAE reduced yield partitioned to position 3 bolls (Table 3). Compensatory increases in yield partitioned on vegetative branches and plants with aborted terminals occurred from 2,4-D exposure2 to 5 and 2 to 6 WAE, respectively. When yield in each position is calculated as a percentage of total hand-harvested yield (Table 4), the NTC partitioned an average of 75%, 16%, 3%, 5%, and 1% of its yield in the first, second, third, vegetative, and aborted terminal positions, respectively. The percentage of yield partitioned in position 1 and 2 bolls was reduced from exposure 2 to 7 WAE. Reduction in percent yield partitioned in position 3 bolls occurred after 2,4-D exposure 2 to 3 WAE (early vegetative growth), whereas an increase in percent yield partitioned to position 3 bolls was observed after exposure 5 WAE (late vegetative growth). Increases in percent yield partitioned to vegetative branches and plants with aborted terminals occurred from 2,4-D exposure 2 to 7 and 3 to 7 WAE, respectively, ranging from early vegetative to early squaring growth stages (Table 4).
The effect of application timing of 2,4-D at 8.3 g ae ha−1 on seed cotton yield partitioning by horizontal position and vertical zone averaged over environment.

a Number of WAE at which application occurred.
b Stage at the time of application.
c Position 1 fruiting sites.
d Position 2 fruiting sites.
e Position 3 fruiting sites.
f Any fruiting sites partitioned on monopodial (vegetative) branches.
g Any fruiting sites partitioned on plants that have lost apical dominance.
h Located on branches from nodes 5 through 8.
i Located on branches from nodes 9 through 12.
j Located on branches from node 13 and beyond.
k Abbreviations: NTC, nontreated check; WAE, weeks after emergence.
* Significantly increased relative to the NTC.
** Significantly decreased relative to the NTC.
The effect of application timing of 2,4-D at 8.3 g ae ha−1 on seed cotton yield partitioning as a percentage of the total treatment weight by horizontal position and vertical zone averaged over environment.

a Number of WAE at which application occurred.
b At the time of application.
c Position one fruiting sites.
d Position two fruiting sites.
e Position three fruiting sites.
f Any fruiting sites partitioned on monopodial (vegetative) branches.
g Any fruiting sites partitioned on plants that have lost apical dominance.
h Located on branches from nodes 5 through 8.
i Located on branches from nodes 9 through 12.
j Located on branches from node 13 and beyond.
k Abbreviations: NTC, nontreated check; WAE, weeks after emergence.
* Significantly increased relative to the NTC.
** Significantly decreased relative to the NTC.
By vertical zone
Seed cotton weight partitioned to zones 1 (nodes 5–8), 2 (nodes 9–12), and 3 (node 13 and higher) is listed in Table 3. Cotton weight partitioned in zone 1 was reduced from 2,4-D exposure 1 to 7 WAE, whereas weight partitioned in zone 2 was reduced from exposure 3 to 8 WAE. Reductions in weight partitioned to zone 3 were observed after exposure of squaring cotton to 2,4-D 6 to 8 WAE (Table 3). When cotton weight is presented as percentage of total weight for each treatment (Table 4), the NTC partitioned 42%, 38%, 14%, 5%, and 1% of seed cotton weight in zones 1, 2, and 3, bolls on vegetative branches, and bolls on aborted plants, respectively. Percent yield partitioned in zones 1 and 2 was decreased after 2,4-D exposure 1 to 6 and 3 to 7 WAE, respectively. Percent yield partitioned to zone 3 was decreased after exposure 6 to 8 WAE and was increased after exposure 4 WAE.
By maturity cohort
Analyzing yield partitioning by fruiting structure age resulted in conclusions similar to the horizontal position and vertical zone analyses. Reductions in yield partitioned to older fruiting sites (i.e., inner positions and lower zones) was generally accompanied by increases in yield partitioned to newer fruiting sites (data not shown).
Fiber quality
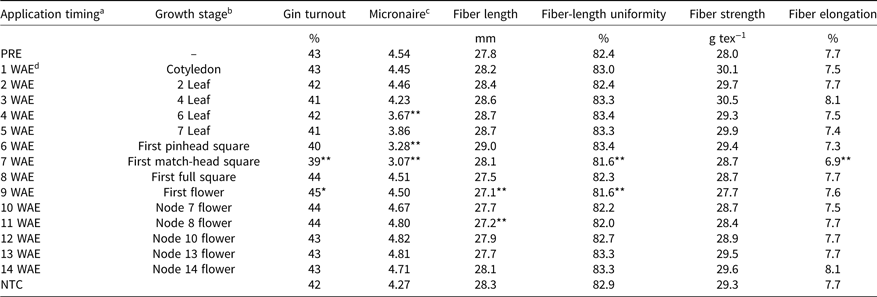
After the observation of delayed maturity in many treatments during the first 2 years of the experiment, an analysis of fiber quality was conducted during the final year. Table 5 lists data on gin turnout, micronaire, fiber length, fiber uniformity, fiber strength, and fiber elongation by treatment averaged over environment. 2,4-D exposure 7 WAE (early squaring) resulted in reduced turnout, whereas exposure 9 WAE (early blooming) resulted in increased turnout. Such effects indicate that seed fraction was increased and decreased, respectively, by 2,4-D exposure just before and after initiation of bloom, a time of physiological stress for cotton. Micronaire was reduced if exposure to 2,4-D occurred 4 or 6 to 7 WAE, and fiber length was reduced if exposure occurred 9 or 11 WAE (early to mid bloom). Fiber-length uniformity was reduced from exposure 7 or 9 WAE, and fiber elongation was reduced after exposure 7 WAE. Overall, small effects on fiber-quality parameters were observed after 2,4-D exposure, with the exception that micronaire was reduced from exposure 4 or 6 to 7 WAE (late vegetative or early squaring growth stages) and fiber-length uniformity was decreased from exposure 7 or 9 WAE (squaring and flowering growth stages). Micronaire >5.0 or <3.4 costs producers because fiber value is discounted (Anonymous 2013) and reductions to fiber-length uniformity of <1% are problematic. Reductions in micronaire after exposure to 2,4-D at 4 or 6 to 7 WAE were likely due to stress to older fruiting structures. Micronaire is altered by environmental stresses such as 2,4-D exposure during the process of fiber-tube cellulose “filling” that occurs after the completion of fiber elongation (Anonymous 2018b). Damage to younger fruiting structures exposed to 2,4-D later in the season likely does not affect micronaire, because fiber-tube filling would not have begun. Conversely, reductions in length could be due to shed of younger fruiting structures present upon exposure 9 or 11 WAE. Because cotton fibers elongate over the course of 15 to 25 days, late-season stress such as 2,4-D exposure may not allow enough time for the plant to recover and elongate properly before harvest (Anonymous 2018b).
Cotton gin turnout, micronaire, fiber length, fiber uniformity, fiber strength, and fiber elongation as affected by application timing of 2,4-D at 8.3 g ae ha−1 averaged over environment.

a Number of WAE at which application occurred.
b Stage at the time of application.
c Score <3.4 or >5.0 indicates poor fiber permeability and qualifies for discounted value; 3.5–3.6 or 4.3–4.9 indicates cotton of base value; 3.7–4.2 indicates cotton of premium value.
d Abbreviations: NTC, nontreated check; WAE, weeks after emergence.
* Significantly increased relative to the NTC.
** Significantly decreased relative to the NTC.
Significance of findings for cotton management
Susceptible cotton cultivars are highly sensitive to dilute concentrations of 2,4-D, consistent with previous findings (Egan et al. Reference Egan, Barlow and Mortensen2014; Everitt and Keeling Reference Everitt and Keeling2009; Johnson et al. Reference Johnson, Fisher, Jordan, Edmisten, Stewart and York2012). Cotton response to 2,4-D is influenced by growth stage at exposure timing. Although this experiment did not consider environment as an experimental factor, previous work has demonstrated that environmental conditions can affect cotton response to auxin-herbicide injury, especially after the exposure event. Byrd et al. (Reference Byrd, Collins, Culpepper, Dodds, Edmisten, Wright, Morgan, Baumann, Dotray, Manuchehri, Jones, Grey, Webster, Davis, Whitaker, Roberts, Snider and Porter2015) reported that although heat unit accumulation may not be pivotal in affecting cotton yield response following 2,4-D exposure, water availability likely is (Byrd et al. Reference Byrd, Collins, Culpepper, Dodds, Edmisten, Wright, Morgan, Baumann, Dotray, Manuchehri, Jones, Grey, Webster, Davis, Whitaker, Roberts, Snider and Porter2015). Thus, the environment and in-season growing conditions are important considerations for maximizing cotton yield and compensatory ability (Anonymous 2018c, File et al. Reference File, Reynolds, Reddy and Arnold2000; Monks et al. Reference Monks, Wehtje, Burmester, Price, Patterson, Delaney, Faircloth and Woods2007; Yasuor et al. Reference Yasour, Sibony, Rubin, Litvak, Negba, Flash and Gat2000). Total lint yield and yield distribution are affected by growth stage at exposure timing. Cotton has the ability to compensate for in-season injury, but delayed maturity and changes in yield partitioning can affect harvest efficacy and fiber maturity (Bednarz and Roberts Reference Bednarz and Roberts2001; Kletter and Wallich Reference Kletter and Wallich1982; Sadras Reference Sadras1995, Reference Sadras1996). Cotton irrigation can help maximize crop resiliency (Anonymous 2018c) and ability to redistribute fruiting structures in response to in-season stress (File et al. Reference File, Reynolds, Reddy and Arnold2000; Monks et al. Reference Monks, Wehtje, Burmester, Price, Patterson, Delaney, Faircloth and Woods2007; Yasuor et al. Reference Yasour, Sibony, Rubin, Litvak, Negba, Flash and Gat2000), which may mask the severity of response to 2,4-D stress that would be exacerbated by water stress had irrigation not been used in this study. Cotton appears to be most susceptible to 2,4-D injury from vegetative to early squaring growth stages. At these stages, cotton is susceptible to yield loss, delayed fruit retention, and consequent changes to partitioning of yield placement after exposure to a sublethal rate of 2,4-D. The response of older, post-bloom cotton to such exposure is generally far less severe, consistent with previous work (Byrd et al. Reference Byrd, Collins, Culpepper, Dodds, Edmisten, Wright, Morgan, Baumann, Dotray, Manuchehri, Jones, Grey, Webster, Davis, Whitaker, Roberts, Snider and Porter2015; Egan et al. Reference Egan, Barlow and Mortensen2014; Johnson et al. Reference Johnson, Fisher, Jordan, Edmisten, Stewart and York2012; Marple et al. Reference Marple, Al-Khatib and Peterson2008). These data show that the time of cotton exposure to 8.3 g ae ha−1 2,4-D is important and that exposure during vegetative or early squaring growth is most likely to affect yield and fiber properties, although fiber analysis was only conducted on samples from two site-years of the experiment.
Author ORCIDs
John T. Buol https://orcid.org/0000-0001-6745-0864; Daniel B. Reynolds https://orcid.org/0000-0002-2607-277X
Acknowledgements
The authors thank Cotton Inc. and Monsanto Co. for partial funding of this research. Representatives from Cotton Inc. and Monsanto Co. are coauthors on this manuscript. No other conflicts of interest have been declared.