


INTRODUCTION
According to Turner (Reference Turner and Gowen1995), water is probably the most limiting non-biological factor affecting banana production. The need for irrigation varies between locations, whilst its justification in commercial terms depends on the purposes for which a crop is grown and its market value. For crops that have international commercial importance, integrated approaches to irrigation research should complement site specific, single discipline, usually empirical methodologies, which are still too common. To avoid duplication of effort, the first need is to collate existing (published) information on the water relations and irrigation needs of individual crops, and to attempt to interpret these data in practically useful ways. Rarely is enough time allocated for this purpose (Carr, Reference Carr, Ferreira and Jones2000).
Such an approach formed the basis for a review paper on coffee (Carr, Reference Carr2001). In a similar way, this paper attempts to review the international literature reporting the results of research on the water relations and irrigation requirements of the banana in an attempt to link fundamental research to irrigation practice, in particular to ensure that water is used as effectively as possible and water productivity is increased (Molden, Reference Molden2007).
First, to facilitate the interpretation and extrapolation of the results of empirical experiments, relevant background information on the origin and centres of production, genetic diversity, development and growth of the cultivated banana is summarized. A comprehensive review of the eco-physiology of bananas has recently been published to which the reader is referred (Turner et al., Reference Turner, Fortescue and Thomas2007). This followed earlier reviews of the environmental physiology of the banana, also by Turner (Reference Turner, Schaffer and Andersen1994; Reference Turner and Arizaga1998).
ORIGIN AND CENTRES OF PRODUCTION
The centre of origin of the wild Musa species, a giant perennial herb, is believed to be in South East Asia, where it opportunistically exploits breaks in the rainforest such as river margins (Simmonds, Reference Simmonds1962). Wild bananas are jungle weeds, pioneers in the succession to rainforest, and intolerant of shade (Price, Reference Price and Gowen1995). From here, the banana is believed to have spread outwards into the Pacific and then westwards reaching sub-Saharan Africa about 2000 years ago (although this conventional view is now being challenged; for example, Lejju et al. (Reference Lejju, Robertshaw and Taylor2006) have identified archaeological evidence of the presence of bananas at Munsa, in Uganda during the fourth millennium BC). The banana became a staple crop in upland East/Central Africa, still the greatest centre of cultivation. In the sixteenth century, early European travellers may have taken the banana from West Africa across the Atlantic Ocean to the Americas where it was quickly adopted (Simmonds, Reference Simmonds, Smart and Simmonds1995).
Bananas can now be found throughout the tropics and subtropics. They are mostly grown between latitudes 30°N and S of the equator, at altitudes up to normally about 1500 m, except in Central and East Africa where some clones are grown up to 2000 m (Stover and Simmonds, Reference Stover and Simmonds1987). In the tropics, they are grown for subsistence and as a cash crop, and play a very important role in diets and in local domestic economies. The fruit can be eaten fresh as a dessert, after cooking, used for brewing, sold in local markets or exported. The leaves and leaf sheaths are variously used as animal feed, to wrap food for steaming, for thatching, for making mats and ropes, and in handicrafts. In these diverse ways bananas support the livelihoods of millions of people (Fleuret and Fleuret, Reference Fleuret, Fleuret, Cattle and Schwern1985).
Commercial cultivation of the crop for export of the fruit to Europe and North America began in the nineteenth century, mostly in tropical America but also to a lesser extent in West Africa (Simmonds, Reference Simmonds, Webster and Wilson1998). Dessert crops grown for export are now found principally in Central and South America, the Caribbean, West Africa (Cote d'Ivoire and the Cameroon) and the Philippines. Ecuador is the world's largest producer for export whilst India, China, Brazil, and the Philippines are the largest producers. Dessert bananas are also grown commercially in the subtropics and in Mediterranean climates including Israel and other eastern Asia countries, for internal consumption or local export (FAOSTAT, 2008). Up to date data are difficult to obtain but, according to Stover and Simmonds (Reference Stover and Simmonds1987), more than two-thirds of the bananas grown in the world for export are irrigated. Robinson (Reference Robinson and Gowen1995, p. 238; Reference Robinson1996) summarized those regions where irrigation is widely practiced including: i) areas of the tropics with pronounced dry seasons, ii) the semi-arid subtropics and iii) Mediterranean environments.
GENOTYPES
Many cultivars of Musa exist, although the genetic base for international banana production is very narrow. They have been selected for diverse agro-ecological areas, and for different culinary purposes. Hybridization is thought to have occurred between various sub-species of M. acuminata and this has led to a range of diploid cultivars. These in turn are believed to have hybridized with M. balbisiana, another diploid species found in the Indian sub-continent (Simmonds and Shepherd, Reference Simmonds and Shepherd1955). The fruits of both these wild ancestors are inedible because they are full of seeds. Triploid cultivars of M. acuminata, and of the hybrids, also occur and these make up the vast majority of cultivated types, including the well-known cultivars now grown for export. Parthenocarpy and the absence of seeds in the fruits are presumed to be the major attributes selected by cultivators. This in turn led to the requirement for vegetative propagation by ‘suckers’ (lateral shoots) and to the development of clones (Simmonds, Reference Simmonds, Smart and Simmonds1995).
The relative expression of M. acuminata (A) and M. balbisiana (B) characteristics and the ploidy level are together used to classify genotypes as, for example, AAA, AAB, ABB (Daniells et al., Reference Daniells, Jenny, Karamura, Tomekpe, Arnaud and Sharrock2001; Purseglove, Reference Purseglove1972; Simmonds, Reference Simmonds, Smart and Simmonds1995; Simmonds and Shepherd, Reference Simmonds and Shepherd1955; Stover and Simmonds, Reference Stover and Simmonds1987;). Although a distinction is frequently made between bananas, a sweet fruit eaten raw, and plantains, a fruit low in sugar and eaten cooked, this distinction is botanically not justified. The term ‘banana’ is now preferred by some as a descriptor for the fruits of all Musa cultivars (Fleuret and Fleuret, Reference Fleuret, Fleuret, Cattle and Schwern1985; Gowen, Reference Gowen1988). The proportion of starch to sugar is reduced as the fruits ripen. This process is slower in the cooking cultivars than in those eaten raw. Some of the cultivar groups with the balbisiana (B) genome are considered to be relatively tolerant of seasonal drought (Price, Reference Price and Gowen1995; Purseglove, Reference Purseglove1972; Simmonds, Reference Simmonds, Smart and Simmonds1995). Although there was apparently no published experimental evidence to support this perception (Turner, Reference Turner and Gowen1995), the results of subsequent laboratory-based leaf gas exchange studies (see below) are consistent with the view that the presence of the B genome contributes to drought tolerance (Thomas et al., Reference Thomas, Turner and Eamus1998).
In recent papers, Ploetz et al. (Reference Ploetz, Kepler, Daniells, Nelson and Elvitch2007) have highlighted the complexity of, and diversity of cultivars within, the Musa genus in the Pacific region alone, whilst Heslop-Harrison and Schwarzacher (Reference Heslop-Harrison and Schwarzacher2007) have reviewed the domestication and genomics of this fascinating crop.
CROP DEVELOPMENT
Vegetative growth
The ‘apparent’ aerial shoot of the banana, known as the pseudostem, is composed of the rolled and enclosing bases of a large number of leaves. This aerial shoot is born on a subterranean stem (rhizome), which grows slowly and horizontally to a length of about 0.3 m. Aerial shoots (suckers or followers) arise from lateral buds on the rhizome. Each shoot is determinate (Norman et al. Reference Norman, Pearson and Searle1984). Mechanically the aerial stem (a sympodium) is completely dependent on the leaf sheaths for support, reaching a height of 2–8 m in cultivated varieties. The actual stem is at or below soil level. The apex initiates the leaf primordia, which develop into leaves that rapidly encircle the shoot apex. The growth in these lateral organs overshadows that in the vegetative apex to create an immense photosynthetic structure. Successive internodes are difficult to discern because of their condensation. This condition changes on flowering when a massive true erect stem forms (Barker and Steward, Reference Barker and Steward1962; Karamura and Karamura, Reference Karamura, Karamura and Gowen1995; Simmonds, Reference Simmonds1966).
The area of individual leaves of dessert cultivars can reach 2–3 m2 and the total leaf area of a plant 17–25 m2 (Stover and Simmonds, Reference Stover and Simmonds1987). In ratoon crops, the leaf area index (L) varies from 2 to more than 6 depending on the cultivar, season and plant density. A value for L of 4.5 is associated with the maximum use of photosynthetically active radiation (Turner Reference Turner1990, quoting others), and corresponds to about 90% of the incoming solar radiation being intercepted by the leaf canopy (Turner et al., Reference Turner, Fortescue and Thomas2007). Splitting of the lamina along the veins is common, but vascular connections between the midrib and the leaf margin remain intact. This tearing of the leaves (into strips <100 mm wide) has been shown to increase the cooling effects of wind, under hot dry conditions, and to increase the efficiency of leaf water use (Taylor and Sexton, Reference Taylor and Sexton1972). More recently, Eckstein et al. (Reference Eckstein, Robinson and Fraser1996) have shown how, in subtropical South Africa, severe leaf tearing (strips 12.5 and 25 mm wide) can result in smaller plants and leaf areas, and a reduction in rates of photosynthesis, together leading to a 22% smaller fruit mass compared to plants with less severe leaf damage.
In Western Australia (25°S), Hoffman and Turner (Reference Hoffman and Turner1993) found that the elongation rate of leaves emerging from the pseudostem (up to 80 mm d−1) of container grown plants (cv. ‘Williams’ AAA Cavendish subgroup) was a sensitive measure of the response of the plant to a drying soil (range soil water potential −10 to −80 kPa).
Inflorescence development
In lowland tropical areas, floral initiation occurs after 30–40 leaves have been produced. This occurs at the apex of the rhizome, which is located within 0.3 m of the soil surface, following which the aerial stem begins to elongate pushing through the centre of the pseudostem until it is visible at the top (a process known as shooting). The floral phase is considered to extend from floral initiation to inflorescence (bunch) emergence from the throat of the pseudostem (the start of the fruiting phase), although the fruit actually exist before they appear external to the plant (Karamura and Karamura, Reference Karamura, Karamura and Gowen1995; Simmonds, Reference Simmonds1966). The flower induction stimulus is not yet known, and flowering can occur at any time of the year,
The inflorescence is a spike with stout peduncles on which flowers are arranged in nodal clusters in two rows on transverse cushions (crown). The first nodes of flowers are female, while the last nodes are male. The fruits grow from the female flowers without pollination (Purselove, Reference Purseglove1972). In cultivated varieties, the inflorescence on emergence behaves geotropically which results in each banana bunch (or stem) hanging in a pendulous position. Mechanically the aerial stem is entirely dependent on the surrounding leaf sheaths for its support.
Holder and Gumbs (Reference Holder and Gumbs1982) reported a study of the effects of the timing of irrigation during floral initiation on female flower production (cv. ‘Robusta’ AAA Cavendish subgroup) on a clay loam soil in St Lucia (14°N). A continuous non-limiting supply of water during the ‘dry’ season from December to July increased the number of flowers produced on the plant crop (planted 1 December, all treatments pre-irrigated). Relieving water deficits after 120 d, for a period of 60 d, during the period of estimated floral initiation and early differentiation had a similar effect, but also increased the number of female flowers per inflorescence compared with the continuously watered treatment. There was evidence of enhanced growth rates (pseudostem girth), for a period of 50 d, following the relief of the water deficit, which made up for the earlier effects of drought. Positive linear correlations were observed between the final (240 d after planting) pseudostem diameter (range 50–58 mm at 0.60 m above the ground) and the number of female flowers per inflorescence (range 100–160; r 2 = 81%, n = 9). Similarly, female flower production was correlated with the rate of increase in the diameter of the pseudostem (1–4 mm d−1) during the period 150–181 d after planting (r 2 = 85%, n = 9).
Fruit growth
The interval between inflorescence (bunch) emergence and harvest is seasonally variable ranging in subtropical South Africa, for example, from 108 d after flowering in early December (summer) to 200 d in early May (autumn), and leading to corresponding uneven fruit production during the year. By tagging inflorescence emergence every two weeks, Robinson and Nel (Reference Robinson and Nel1984) found that it was possible to predict harvest dates based on historical records. There were also differences in bunch mass depending on the time of flowering, linked to the minimum temperatures prevailing at flower initiation. For example, Robinson (Reference Robinson1982), again in South Africa, reported how inflorescences that emerged from plants in November produced bunches, which were small and malformed. This was explained as the effect of low temperatures at the time the flowers were being initiated in June.
In the sub-tropics, an individual mean bunch mass of 50 kg is possible from ratoon crops (cv. ‘Williams’ AAA Cavendish subgroup,). By comparison the corresponding weight in the tropics is 30–35 kg (Robinson and Nel, Reference Robinson and Nel1989). A bunch contains a cluster of fruits at a node (known as a hand), which in turn is composed of individual fruits (or fingers). The effects of drought at this time are illustrated by the results of an experiment in the Canary Islands (28°37′N). When water was withheld for 63 d from flower emergence before re-watering (cv. ‘Grande Naine’ AAA Cavendish subgroup) finger number remained constant (not surprisingly) compared with the control, but finger length and diameter were both reduced (by 9%). Total bunch fresh weights were reduced by 41%, from 30 to 17 kg plant−1. Drought also delayed fruit maturity (Mahouachi, Reference Mahouachi2007).
Root developmentFootnote 2
The subterranean parts of the bananas follow the same overall arrangement as many other monocotyledons. Arising from the upper parts of the rhizome are the root axes (nodal roots, also known as cord roots) that produce primary (first order) laterals from which may develop secondary (second order) laterals. An axis with its laterals is considered to be a root. A single shoot can produce several hundred roots (Price, Reference Price and Gowen1995). Root hairs up to 2 mm in length occur behind the root apex. Cord roots are relatively straight and cylindrical reaching lengths of 3–5 m, and diameters of 4–10 mm (Draye et al., Reference Draye, Lecompte, Pages, Turner and Rosales2005). In South Africa, Robinson (Reference Robinson1987) found that primary laterals remained functional (based on appearance) for about eight weeks, secondary laterals for five weeks and root hairs for three weeks. Roots are produced continuously until flowering.
In the Jordan Valley of Israel (ca. 32°N; alt. −210m), early studies of the roots of banana (cv. ‘Dwarf Cavendish’ AAA Cavendish subgroup) were reported by Shmueli (Reference Shmueli1953). Using trenches and a water jet to wash away the soil, and direct core sampling, a dense mass of, mainly horizontal, roots was recorded from a depth of 0.02 m down to 0.4–0.45 m. There was then a sharp decrease in the number of roots, with a few vertical roots below 0.6 m, but with some extending to 0.7–0.8 m by the time fruit was forming. Roots of suckers with 13–14 visible leaves reached depths of about 0.3 m. Roots extended laterally up to 3.3 m from the mother plant and sucker. Secondary roots of two types, depending on diameter and length, formed only on primary roots at least 0.2 m in length. The soil was high in calcium carbonate (35–55%) with a combined clay plus silt fraction of 55–75%. The crop was irrigated and the water table was below 3 m depth at all times. The soil was mulched and not cultivated.
In South India (11°00′N alt. 420 m), Krishnan and Shanmugavelu (Reference Krishnan and Shanmugavelu1980) studied the effects of three irrigation regimes on root distribution (cv. ‘Robusta’ AAA Cavendish subgroup). The maximum depth of rooting, observed at harvest, was similar in all three treatments (ca. 0.7 m), whilst the corresponding lateral spread was about 3 m. Infrequent irrigation resulted in slightly deeper and wider root systems than were found with more frequent applications of water. There were no effects of irrigation regime on the dry mass of roots, or on the total root number or length. Root depths at the time of shooting were similar to those observed at harvest, but lateral spread was 0.5–0.6 m less.
In New South Wales, Australia (28°50′S), Trochoulias and Murison (Reference Trochoulias and Murison1981) found that 70% of the roots (live cord roots with diameters greater than 1 mm counted in 0.2 × 0.2 m squares on an exposed soil profile) were concentrated in the top 0.4 m of a clay loam soil, regardless of the supplementary (drip) irrigation treatment. In addition, 40% of the root system of 10–12 month old plants (cv. not specified) was found in a 0.6 × 0.6 m square close to the base of the plant.
In the northern coastal plain of Israel (33°16′N), Lahav and Kalmar (Reference Lahav and Kalmar1981) compared the effects of several drip irrigation treatments on root growth by counting the number of root cords exposed on a brown vertisol soil. In all cases, root distribution (cv. ‘Williams’ AAA Cavendish subgroup) was uniform at distances up to 2.5 m from the planting station (or mat). Roots extended to maximum depths of nearly 1.0 m, with 75% in the top 0.6 m.
Summarizing results of root studies in South Africa, Robinson (Reference Robinson1996) stated that 88% of the primary roots were at 0–0.3 m depth (cv. ‘Williams’ AAA Cavendish subgroup), 9% from 0.3–0.4 m and only 3% below 0.4 m. Water was extracted mainly (87%) from the top 0.3 m of soil when irrigated (Robinson and Alberts, Reference Robinson and Alberts1989). The ‘effective’ rooting depth was considered to be only 0.3–0.4 m. By contrast, Daniells (Reference Daniells, Cull and Page1986) in northern Queensland (17°38′S) found that, although roots (cvs ‘Williams’ AAA, and ‘Corne Plantain’ AAB) extended to depths of 0.6 m in an alluvial clay loam soil, water was extracted from 0.9 m (the limit of measurement, with tensiometers) and from within 1.5 m of the stem.
In a detailed study designed to establish guidelines for irrigation water management of bananas (cv. ‘Pacovan’ AAB Prata subgroup) in north-east Brazil (9°9′S alt. 365 m), root distribution was evaluated over a 33-month period using the soil profile method supplemented by digital image analysis (Bassoi et al., Reference Bassoi, Moura e Silva, Gomes da Silva, Ramos and Sediyama2004a). The ‘effective’ rooting depth (embracing 90% of the total length of roots > ca. 1.0 mm diameter), in a medium textured latosol soil, increased from 0.40 m at three months after planting to about 0.60 m after one year, 80 days after the end of flowering, when the rooting depth was about 1.0 m (the maximum depth of observation). Roots reached the mid-way between plants (spaced 3.0 m apart) six months after planting. Total root length increased throughout the period of observation, but at a declining rate. The recommended soil depth for monitoring and scheduling irrigation at this site was 0.40 m for the first nine months from planting and afterwards at 0.60 m with the instrumentation installed 0.60 m away from the stem.
In Costa Rica (10°12′N alt. 268 m), Araya et al. (Reference Araya, Vargas and Cheves1998) and Araya (Reference Araya, Turner and Rosales2005) compared the effects of several factors on root distribution of two cultivars (‘Valery’ and ‘Grande Naine’ both AAA Cavendish subgroup) grown in commercial banana plantations. Root fresh weight decreased sharply with soil depth independent of distance from the pseudostem with more than 65% being found in the 0– 0.30 m depth increment. The roots of ‘vigorous’ plants reached depths of 1.2 m and those of ‘poor vigour’ 0.75 m.
In southeastern Nigeria (4°42′N alt. 10 m), Blomme et al. (Reference Blomme, Teugels, Blanckeart, Sebuwufu, Swennen, Tenkouano, Turner and Rosales2005) reported that ‘most roots’, as observed by core sampling of four cultivars, were to be found within a 0.60 m radius of the plant and to depths of about 0.70 m. Previously, Blomme and Ortiz (Reference Blomme, Ortiz, Craenen, Ortiz, Karamura and Vuylsteke2000) had compared the root systems of 11 genotypes from six diverse Musa groups at the same high rainfall site. There was considerable variability in root development both between and within the groups. Most genotypes had the majority of roots in the 0–0.15 m layer, and no roots were found below 0.8 m.
In a controlled environment experiment in the UK, Kalorizou et al. (Reference Kalorizou, Gowen and Wheeler2007) found that resistance to nematodes (a major constraint to banana reduction in some places as a result of the damage they cause to primary roots) was associated with two clones (AAA and AABB) with greater root mass and more and larger primary roots than the other five cultivars tested. In Uganda (5°13′N alt. 1200 m), Kashaija et al. (Reference Kashaija, McIntyre, Ssali and Kizito2004) found that legume intercrops had no effect on the vertical and horizontal distribution of roots of banana (AAA), or nematodes. Approximately 90% of the root biomass was in the upper 0.30 m whilst there was none below 0.70 m. Within 0.50 m of the banana ‘mat’, the majority of the root mass was in the surface 0.15 m but outside this radius more were found at depths from 0.15–0.30 m. In a review, Delvaux (Reference Delvaux and Gowen1995) confirmed the sensitivity of banana roots to physical constraints as they rarely explore compacted soils. For example, on a range of soils in Martinique (ca. 14° 47′N), root density, defined as the number of roots per unit of soil surface, increased by a factor of about six as the dry bulk density declined from about 1.2 to 0.7 g cm−3.
Robinson and Bower (Reference Robinson and Bower1988) recorded seasonal root growth (cv. ‘Williams’ AAA Cavendish subgroup) over a 12-month period in an underground root laboratory in Nelspruit, South Africa (25°28′ alt. 700 m). In this sub-tropical region, maximum extension rates of primary roots were observed in late summer (mean 160, maximum 275 mm week−1) before declining during the autumn. In the tropics (Ivory Coast; 5°37′N alt. 78 m), Lassoudiere (Reference Lassoudiere1978) observed similar peak rates of root extension. Extension ceased completely in the winter when soil temperatures, at 0.2 m depth, were 10–13 °C (at 08:00 hours). Leaf development was continuing at this time at about one leaf month−1, compared with five leaves month−1 in the summer. Root hairs developed on primary roots after about one week and continued growing for a further three weeks after which they died back. In a subsequent paper, Robinson and Alberts (Reference Robinson and Alberts1989) illustrated a very highly significant relationship (r2 = 84%; n = 43) between root extension rates and soil temperature (over the range 11.5–25 °C) recorded at a depth of 0.2 m (at 08:00 hours). Extension rates were erratic at temperatures above about 22 °C. Although the links are tenuous, these differences in seasonal root activity were thought to explain, at least in part, corresponding differences in transpiration rates and irrigation need.
As Draye et al. (Reference Draye, Lecompte, Pages, Turner and Rosales2005) observed ‘the volume of soil where the uptake of water and nutrients occurs is constantly changing. . . Unfortunately, these time related components of root distribution remain poorly addressed.’ Detailed quantitative studies of the root system of the banana have, however, been undertaken and reported by Lecompte and his co-workers in Guadaloupe (15°09′N alt. 485 m) in order to facilitate the development of models of root system architecture (e.g. Lecompte et al., Reference Lecompte, Vaucelle, Pages and Ozier-Lafontaine2002; Lecompte and Pages, Reference Lecompte and Pages2007).
Conclusions
Almost regardless of the method of root observation employed, it appears that roots of banana can:
• Spread laterally 2–3 m from the pseudostem, and sometimes up to 5 m. However, most roots are usually found within 0.6 m of the base of the plant.
• Extend to depths of 1.0–1.5 m, providing that there are no physical restrictions. Relatively few are found below 0.6–0.8 m. Root extension virtually ceases at flowering.
• The ‘effective’ depth of rooting (however defined) is often taken to be 0–0.40 m, sometimes extending to 0.60 m.
• In the subtropics, root growth is seasonal, and temperature dependent.
• It appears that irrigation has only a small effect, if any, on the size and distribution of the root system.
• There is some (limited) evidence that small differences between cultivars may exist. This needs to be explored further ‘particularly for non-commercial cultivars grown in subsistence agriculture’ (Price, Reference Price and Gowen1995).
PLANT WATER RELATIONS
Robinson and Bower (Reference Robinson and Bower1987) commented that, despite the sensitivity of bananas to water deficits, there was very little published work on the physiological indicators of these deficits. This was due, in part, to difficulties in measurement, the presence of latex and the very efficient stomatal regulation of transpiration, first reported by Shmueli (Reference Shmueli1953) in Israel. Subsequently, Turner and Thomas (Reference Turner and Thomas1998) showed how measurements of the volumetric (relative leaf water content) or thermodynamic tissue water status (leaf water, osmotic and pressure potentials) of a laticiferous plant like the banana, using a range of traditional methods do not help to explain gas exchange processes. In a short-term pot experiment in Western Australia (32°S), they found a better association between stomatal conductance and net photosynthesis with soil water potential, over the range −1 to −60 kPa, than with leaf water status. The Scholander pressure chamber technique for measuring leaf water potential is not suitable for use with the banana because of the difficulty of distinguishing the exudation of xylem sap from that of the latex. The method described by Milburn et al. (Reference Milburn, Kallarackal and Baker1990), which is based on measurements of the refractive index of exuded latex, was preferred and its reliability subsequently confirmed by Thomas and Turner (Reference Thomas and Turner2001). Some changes in the osmotic components (30%) of leaf water potential were observed during the day but differences caused by drought, in the leaf and the root, over the five days were small. The water potential of well-watered plants was found to cycle diurnally within the remarkably narrow range of 0 to –0.35 MPa. In fact, the rate of extension of the youngest leaf may be the most sensitive indicator of plant water status (Kallarackal et al., Reference Kallarackal, Milburn and Baker1990), providing it is not too hot (Thomas and Turner, Reference Thomas and Turner1998). Under hot, arid conditions, leaf folding is not considered to be a reliable plant-based indicator of when to irrigate (Thomas and Turner, Reference Thomas and Turner1998).
Stomatal behaviour
Although stomata are present on both the adaxial (upper) and abaxial (lower) surfaces of the leaf, their density is up to four times greater on the lower (150–170 mm−2) than the upper surface (35–50 mm−2) (Brun, Reference Brun1961; Chen, Reference Chen1971). In subtropical South Africa (25°7′S), Eckstein and Robinson (Reference Eckstein and Robinson1995a) found that the density of the stomata on either surface (ca. 130/54 mm−2 respectively) was not affected by the season (cv. ‘Grand Naine’ AAA Cavendish subgroup).
In pioneering studies in the Jordan Valley of Israel (ca. 32°N alt. −210m), Shmueli (Reference Shmueli1953) estimated relative stomatal opening using the infiltration liquid method (based on kerosene) to try and identify the optimum irrigation interval. Measurements were made on the third fully expanded leaf, counting from the top, exposed to sunlight on plants (cv. ‘Dwarf Cavendish’ AAA Cavendish subgroup) irrigated at intervals of either five or about 10 days. In addition, one plot was allowed to dry to permanent wilting point. The relative infiltration index was first checked against direct microscopic measurement of stomatal apertures.
During the first four days after irrigation the stomata, on both leaf surfaces, remained wide open throughout most of the day. Partial closure began a few hours before sunset. Stomata on the upper surface were usually wider open than those on the lower surface. When about one-third of the available water was depleted there was a gradual reduction in the degree of stomatal opening from midday or earlier, with stomata on the lower surface closing first. When the available soil water was depleted by about two-thirds the pattern of opening of the stomata changed again. There was then one low peak early in the morning followed by a slow decline in the degree of opening during the rest of the day. Stomata on both surfaces of the leaf then behaved in similar ways.
Measurements were also made on one day in a similar crop watered by flood irrigation. The pattern of stomata opening was observed to differ from that of a sprinkler irrigated crop. In particular, stomata on the lower leaf surface were wider open than those on the upper surface, at all three levels of available soil water tested. Measurements made between 12:00 and 13:00 hours showed clearly how the stomata began to close, in both sprinkler and flood irrigated crops, when about 20% of the available water in the 0.9 m deep soil profile had been depleted.
Stomata on leaves shaded from the sun were always wider open on the lower surface than the upper one, the opposite response from that observed on sunlit leaves. The diurnal pattern of opening was also different, and these stomata were generally less sensitive to changes in soil water status than those on leaves exposed to the sun.
In Taiwan (ca. 24°N), Chen (Reference Chen1971) found that stomata were always closed at night, but began to open at dawn reaching maximum apertures in the mid-morning before starting to close during the afternoon with complete closure by 18:00 hours. On cloudy days the same pattern was followed but the maximum apertures reached were less than half those recorded on sunny days. Ke (Reference Ke1979) reported the results of a similar study, also in Taiwan, with similar findings. The stomata opened early in the morning and continued to open as the light intensity increased until about noon when they began to close rapidly, regardless of light intensity, with full closure by 18:00 hours throughout the year. Stomata on the abaxial leaf surface tended to open quicker in the morning and to remain open longer during the day than those on the adaxial surface. The stomata were sensitive to changes in soil water availability.
In subtropical South Africa, Robinson and Bower (Reference Robinson and Bower1988) reported that stomatal conductances of well-watered plants (cv. ‘Williams’ AAA Cavendish subgroup), at midday and in full sunshine, were about four times greater on the lower surface than the upper one (2.26 ± 0.07 and 0.57 ± 0.04 cm s−1 respectively). There was a similar difference in the relative partitioning of transpiration from the upper and lower surfaces of the leaf (see below).
Photosynthesis
In South Africa, Eckstein and Robinson (Reference Eckstein and Robinson1995a) showed that maximum physiological activity, including photosynthesis, occurred in fully expanded leaves, numbers two to five (cv. ‘Grand Naine’ AAA Cavendish subgroup), counted from the top of 1.1 m tall plants (the maximum leaf number at the time of measurement was nine). No differences in activity (photosynthesis, transpiration or stomatal conductance) could be discerned between measurements made in the proximal, medial and distal third of leaves two to five. It was concluded that any measurement point on these leaves could therefore be considered to be representative of the entire leaf. The photosynthetic potential of these leaves was however suppressed during winter months at this subtropical site (25°7′S alt. 720m).
The decline in rates of photosynthesis in leaves six to nine, by up to 38% relative to the maximum, indicated the relatively short life span of the photosynthetic apparatus in banana, a C3 species. The rate of photosynthesis of the youngest leaf that is proximal to the bunch was also low. Although green leaf pruning is not recommended as a management technique, a standard practice in the subtropics is to remove the lower leaves (those hanging below the horizontal) in order to increase light penetration, pseudostem temperature and leaf emergence rate, and to reduce the ratoon cycle time (Robinson et al., Reference Robinson, Anderson and Eckstein1992).
Eckstein and Robinson (Reference Eckstein and Robinson1995a) also found that photosynthesis rates were reduced by unfavourable climatic conditions in the autumn and spring, and more on the adaxial surface than on the abaxial surface of the leaf. In the summer, photosynthetic rates were at their highest, since leaves three to five were replaced every month. The cessation of leaf production after flowering and the ageing of the leaves meant that photosynthesis rates then declined, especially during the last two months of bunch development. In a companion paper, Eckstein and Robinson (Reference Eckstein and Robinson1995b) described the influence of weather variables on seasonal and diurnal changes in gas exchange processes. In the summer, photosynthesis peaked during the morning, and in the afternoon large saturation deficits of the air, up to 3.5 kPa, (and high leaf temperatures, 35–40 °C) resulted in partial stomatal closure and reduced rates of photosynthesis. In the winter, low night temperatures (as low as 6 °C), large saturation deficits (although very unlikely?) and a depleted root system were considered to be the main reasons for low physiological activity at this time of the year.
Eckstein and Robinson (Reference Eckstein and Robinson1996) believed that reductions in photosynthesis, as a result of water stress, were the result of both stomatal limitations (84%) and a ‘disturbed photosynthesis reaction’ (13% higher internal concentration CO2). The physiological responses of tissue cultured plants (cv. ‘Williams’ AAA Cavendish subgroup) to different irrigation treatments were monitored using measurements of leaf gas exchange. During the autumn, the first signs of water deficit appeared after four days of water shortage. After 12 days, there was a 79% reduction in photosynthesis relative to the irrigated (daily) control treatment. Physiological recovery of the plant from short-term water deficits took longer than three days. To maintain leaf gas exchange rates, the soil water potential (Ψm) should be maintained above –15 to –20 kPa, and irrigation intervals should not be longer than three days. Water shortages in the winter were less severe on assimilation than during warmer seasons.
In Western Australia (32°S), Turner and Thomas (Reference Turner and Thomas1998) measured rates of photosynthesis of pot-grown plants (cv. ‘Grand Naine’ AAA Cavendish subgroup) in a glasshouse over a five-day period. The photosynthetic photon flux density was typically below 800 μmol quanta m−2 s−1 (range 400–1400) and net photosynthesis rates, under relatively mild conditions, for irrigated plants were in the range 8–10 μmol quanta m−2 s−1. Drought reduced net photosynthesis when Ψm < −33 kPa and there was no leaf gas exchange at −62 kPa. This was despite there being few, small differences in the leaf water status between irrigated and droughted plants due to the high levels of hydration of banana leaves. Net photosynthesis was proportional to stomatal conductance, both variables being influenced by the photon flux density as well as by the drying soil. Raising the carbon dioxide concentration of the ambient air to 1600 μl l−1 increased net photosynthetic rates from 10 to 15 μmol CO2 m−2 s−1 in irrigated plants and from 0.2 to 2.0 μmol CO2m−2 s−1 in droughted plants, indicating to the authors that non-stomatal inhibition of photosynthesis was not important. However, following a series of field and pot experiments conducted at two sites in Western Australia (16°S and 32°S), the same authors subsequently concluded, based on chlorophyll fluorescence and photosynthesis measurements, that it was a combination of stomatal and non-stomatal factors that reduced net photosynthesis in droughted plants (Thomas and Turner, Reference Thomas and Turner2001).
In a similar short-term field experiment to the one described above, but this time under hot, arid conditions, Thomas and Turner (Reference Thomas and Turner1998) again compared leaf exchange processes of irrigated and droughted plants (cv. ‘Williams’ AAA Cavendish subgroup). At this site in Western Australia (16°S alt. 50 m), where air temperatures are commonly >35 °C and saturation deficits >4 kPa, they found that a single curve related photosynthetic rates to stomatal conductances for both droughted and frequently irrigated (daily) plants. With photosynthetic photon flux densities typically above 1000 μmol quanta m−2 s−1, net photosynthesis rates, under these extreme conditions (Epan = 10 mm d−1) were in the range 15–20 μmol quanta m−2 s−1 for irrigated plants. Net photosynthesis was reduced when Ψm fell below −30 kPa (at 0.30 m depth) and in irrigated plants when the saturation deficit of the air exceeded about 4.5 kPa.
Transpiration
In the Jordan Valley of Israel, Shmueli (Reference Shmueli1953) attempted to measure transpiration using a sensitive balance to record changes in weight of leaf sections taken from field grown plants. This early work suggested that transpiration reached a peak in early to mid-morning and then declined during the rest of the day. Sometimes there was a second peak later in the afternoon. Transpiration rates declined earlier in the day in plants where the available soil water content was below two-thirds of the total. There was no relationship between transpiration and the degree of stomatal opening. High rates of transpiration were recorded even when the stomata were apparently partially closed.
In Taiwan, Chen (Reference Chen1971) also attempted to measure transpiration rates on a diurnal basis using a self-made automatic recorder, and found that the rates tended to follow the same trends as those reported above for stomatal opening, with peak rates occurring around midday on sunny days.
In a carefully designed and monitored experiment, Robinson and Bower (Reference Robinson and Bower1987) compared transpiration rates, measured with a continuous flow steady state Licor porometer from plants (cv. ‘Williams’ AAA Cavendish subgroup) growing in containers in a fibreglass tunnel in the Eastern Transvaal in South Africa (25°7′S alt. 720m). They created two water regimes, soil re-wetted to field capacity daily and continuous drying, and mild (0.4–0.6 kPa) and enhanced (1.5–2.0 kPa) saturation deficits of the air. The photosynthetically active radiation levels inside the shelter were about 45% of those in the open. With humid air there was little difference in transpiration rates between the two water regimes until the soil was relatively dry (Ψm < −80 kPa at 0.2 m depth). By contrast, when the air was dry, transpiration rates from unirrigated plants fell below those from those watered daily when Ψm reached about −20 kPa, two to three days after watering ceased, and then declined rapidly as the soil continued to dry. The coefficients of variation for measurements made on well-watered plants were always low (ca. 10%) but very large (ca. 100%) in droughted plants, with individual measurements showing much variability, despite precautions. This was thought to be due to stomatal cycling.
In an associated field experiment, diurnal measurements of transpiration were made on a plant crop of the same cultivar over a 14 d period without any rain, after wetting the soil profile to field capacity. The control treatment was watered each evening. Peak transpiration rates were two to three times greater than those recorded in the shelter (26 and 10 μg cm−2 s−1 respectively). Transpiration rates followed a diurnal trend, usually peaking in early or mid-afternoon. Differences in transpiration between the two watering treatments first became evident when the saturation deficit of the air exceeded about 2.3 kPa. Transpiration from the unirrigated plants fell below those watered daily within three days of the treatments being imposed, when Ψm, at a soil depth of 0.2 m, was between −20 to −25 kPa. For a clay loam soil with an available water capacity of about 150 mm m−1, this corresponded to less than 25% depletion of the available water in the 0.3 m deep root zone,
Stomatal conductance was found to be an even more sensitive indicator of plant water status than transpiration, with values declining rapidly as the soil dried below field capacity. There was a 50% reduction in conductance when Ψm reached −65 kPa, which corresponded to a 54% depletion of the available water. The prevailing saturation deficit of the air at this time was 2.1 kPa. By comparison the corresponding reduction in transpiration rates was about 30%. When Ψm fell to −525 kPa (73% depletion), stomatal conductances in the unwatered plants were reduced to 82% of those in plants watered daily, and transpiration to 70%. This was 14 d after differential treatments had been imposed. Leaf temperature was not a very sensitive indicator of water deficit, with a corresponding temperature difference of only 2 °C.
As a result of these observations Robinson and Bower (Reference Robinson and Bower1987) recommended that bananas, in this part of the subtropics, should be irrigated at intervals of one or two days only, depending on the prevailing evaporation rates, at a soil water deficit of only 10 mm. This is a value far less than those recommended for virtually any other field grown crop.
The above paper was exceptional in that it specified clearly the sampling procedures used for measurements. An associated paper by the same authors (Robinson and Bower, Reference Robinson and Bower1988) described in more detail how the measurement techniques for transpiration and stomatal conductance were standardized to minimize plant-to-plant variability (coefficient of variation only 5%). Measurements were then made on plants (cv. ‘Williams’ AAA Cavendish subgroup) of uniform size and height (1.5 m tall, plant crop), sequentially planted and watered daily. Diurnal trends in stomatal conductances and transpiration rates were monitored on the abaxial surface of the proximal third of the third, fourth, and fifth youngest leaf, angled towards the sun, on cloudless days, during different seasons in the Eastern Transvaal. Similar measurements (cv. ‘Dwarf Cavendish’ AAA Cavendish subgroup) were also made on one day at a site in South Eastern Transvaal (25° 30′S alt. 369 m), where evaporation rates were higher than at the main research station. Seasonal trends in transpiration were also observed.
During the spring and summer the stomata were apparently wide open from 08:00 to 16:00 hours, before starting to close as radiation levels declined. In the autumn there was a similar trend, but peak conductances were less than a half of those recorded in the summer, and declined even further in the winter when plant-to-plant variability was also greatest.
By comparison, transpiration rates increased gradually from 07:00 hours and peaked at 13:00 hours in the autumn, or at 16:00 hours in the summer, before declining rapidly, especially in the summer. Under high evaporation rates, transpiration rates peaked earlier in the day (11:00 hours) before declining from 14:00 hours onwards. Cumulative transpiration from selected leaves ranged from the equivalent of 1.8 mm d−1 in the winter to 8.7 mm d−1 in the summer. Ambient air temperatures reached maximum values of 27.4, 33.4, 29.6 and 21.8 °C in the spring, summer, autumn and winter respectively, and 37.2 °C at the second site, on the days that measurements were made. Leaf temperatures were close (within 1 °C) to the ambient air temperature during the spring, summer and autumn, but exceeded air temperature by 3–4 °C in the winter, and in the summer at the site with high evaporation rates.
Diurnal cumulative transpiration rates expressed as a function of daily evaporation from a USWB Class A pan varied between seasons, from about 0.97 mm mm−1 in the summer down to 0.61 mm mm−1 in the winter. This difference was explained in part by variability in the responses of transpiration to diurnal changes in the saturation deficit of the air depending on the season. Thus in the spring, summer and autumn transpiration increased with the saturation deficit up to values of about 1.5 kPa. The response curves then diverged, and it was only on summer days that transpiration continued to increase as saturation deficits rose to about 3.5 kPa. In the winter, transpiration rates were low at all saturation deficits, but increased linearly over the range 0.5–1.7 kPa. These contrasting responses were explained in part by observed seasonal differences in root activity: root extension, for example, ceased in the winter months (see above). The results highlight the sensitivity of bananas to evaporative demand for water in relation to the rate of supply from the soil to the leaf, even when the soil water content is close to field capacity.
In a short-term study of leaf gas exchange processes in a hot arid site in Western Australia (16°S alt. 50 m), Thomas and Turner (Reference Thomas and Turner1998) found that transpiration, in contrast to photosynthesis, increased for well-watered plants of the same cultivar (Williams) with the saturation deficit of the air (range 1.8–5.5 kPa), but declined for ‘droughted’ plants when the saturation deficit exceeded about 3–4 kPa.
Cultivar comparisons
In a comparison of 17 Musa spp. genotypes in Ibadan, Nigeria (7° 30′ N alt. 210 m), Ekanayake et al. (Reference Ekanayake, Ortiz and Vuylsteke1994) identified, on the basis of leaf conductance measurements, two ABB cultivars (‘Fougamou’ and ‘Bluggoe’) that were potentially tolerant of transient dry conditions, and two others that were very sensitive to short dry spells (‘Bobby Tannap’ AAB and one of its hybrids TMP×582–4). Later, the same authors, compared leaf stomatal conductances and morphology of 18 genotypes at two contrasting sites in Nigeria (Omme 4°43′N alt. 3 m; Ibadan 7°30′N alt. 210 m). Significant interactions, for example between clone and location, clone and sampling time, suggested that conductance and transpiration of a specific clone needed to be considered for a given environment for useful conclusions to be reached. In general, Ekanayake et al. (Reference Ekanayake, Ortiz and Vuylsteke1998) concluded that ABB genotypes had higher conductances than other taxonomic groups (AAB, AA, AAA and AAAB), and that resistance to black sigatoka leaf spot disease is not due to differences in stomatal morphology or physiology.
In a laboratory based, pot study in Darwin, Australia Thomas et al., (Reference Thomas, Turner and Eamus1998) compared the effects of environmental variables on leaf gas exchange processes (including transpiration) of three cultivars differing in their genomic constitution (‘Williams’ AAA; ‘Lady Finger’ AAB; ‘Bluggoe’ ABB). They found that, as the saturation deficit of the air was increased (from 1.5 to 5.7 kPa), both stomatal conductance and net photosynthesis declined linearly. Since increasing proportions of the B genome reduced this sensitivity to the dryness of the air and increased the instantaneous water use efficiency of the leaf, Thomas et al. (Reference Thomas, Turner and Eamus1998) concluded that the B genome contributes to drought tolerance in Musa spp.
Conclusions
• Stomata are present on both surfaces of the leaf: densities (and conductances) are up to four times greater on lower surface than upper surface.
• Stomata are closed at night; peak opening is reached by midday sometimes followed by progressive closure.
• The degree of stomatal opening is a very sensitive indicator of soil water availability and plant water status.
• Reductions in photosynthesis as a result of water deficit are mainly due to stomatal limitations to gas exchange.
• To maintain gas exchange rates the soil water potential should not fall below −15 to −33 kPa (at 0.2–0.3 m depth), leading to recommendations that irrigation intervals should not exceed three days.
• Transpiration rates can be limited by dry air (e.g. when saturation deficits exceed 2.0–2.3 kPa).
• In the subtropics, there are seasonal differences in the sensitivity of transpiration rates to the dryness of the air and evaporative demand, thought, in part, to be due to differences in root activity.
• As a result, cumulative transpiration, expressed as a proportion of USWB Epan, can vary from 0.61 in the winter to 0.97 in the summer.
• There is some (limited) evidence that the presence of the B genome contributes to drought tolerance (as indicated by measurements of gas exchange).
CROP WATER REQUIREMENTS
Rainfall interception
Harris (Reference Harris1997) reported the results of measurements of rainfall partitioning by a banana canopy (cv. ‘Robusta’ AAA Cavendish subgroup, first ratoon) in St Lucia in the Windward Islands in the eastern Caribbean (ca. 13°54′N). Over a three and a half month period there were 28 rainfall events totalling 723 mm of rain. Both through-fall and stem-flow were highly correlated with rainfall amount and accounted, on average, for 80 and 10% respectively, of incident rainfall. The balance of 10% was assumed to have been intercepted and to have been lost to the atmosphere by evaporation. The volume of water reaching the base of the pseudostem was considered to be about 13 times larger than would be expected on a proportional plan area basis. The spatial distribution of the water passing through the canopy changed with time and the age of the plants. These results are important when considering the water balance of a crop, including irrigation scheduling, and nutrient placement beneath the canopy, but are rarely taken into account. Recently, this issue has started to be addressed in Guadeloupe. Based on detailed measurements of rainfall interception processes and the partitioning between splash and storage of raindrops differing in drop diameter, kinetic energy and fall height, empirical relationships were developed for the application of a rainfall interception model to simulate water flows beneath banana plants (Bassette and Bussière, Reference Bassette and Bussière2008).
Evapotranspiration
Over the past 40–50 years, many different methods have been used to determine the actual water use of the banana plant, including those based on the water balance approach. These involve, for example, measurements of changes in soil water content and/or the use of lysimeters. Most recently, attempts have been made to measure sap flow directly. Estimates of evapotranspiration, or transpiration alone, are then linked to direct measurements of evaporation from, commonly, a USWB Class A evaporation pan, or estimates of potential evaporation using weather data in order to develop a pan or crop factor (usually represented by Kc). All estimates are subject to large errors, and can be locally site specific. This topic is reviewed under three ecological headings, tropics, subtropics and Mediterranean climates.
Tropics
In the Upper Aguan Valley in Honduras (ca. 15°22′N alt. 250 m), an area where the banana is widely irrigated, Arscott et al. (Reference Arscott, Bhangoo and Karon1965) attempted to develop a method of determining the water requirements of the cv. Giant Cavendish (AAA Cavendish subgroup). Based on measurements of changes in soil water content (volumetric) over a one-year period they developed a multiple regression equation (without standard errors) relating daily crop water use to mean air temperature and relative humidity. Actual measured rates of water use for irrigated crops ranged from about 5.7 to 9.2 mm d−1. Interestingly they reported that when ‘hot dry winds’ prevailed rates of water use declined. This they associated with the dryness of the air (saturation deficit) causing transient wilting whenever potential transpiration rates exceeded the capacity of the plants to supply water from the soil to the leaf surface. This tended to occur in those months when the mean air temperatures were about 28 °C and the relative humidity of the air, recorded on five occasions during each day (07:00, 09:00, 12:00, 15:00 and 17:30 hours) with a sling psychrometer, averaged about 63%. This corresponds to a saturation deficit value for the air of about 1.5 kPa.
Subsequently Ghavami (Reference Ghavami1973), in the irrigated Sula Valley of Honduras (ca. 15°20′N alt. 30m), used non-weighing, drainage lysimeters (2.1 m deep), with the soil surface protected from rainfall, to determine the actual water use of bananas (cv. ‘Valery’ AAA Cavendish subgroup). Cumulative monthly evapotranspiration (ETc, mm), from a well-watered group of mature and immature plants, was linearly related (r = 0.93; n = 12) to cumulative evaporation from a USWB Class A pan sited (conventionally) in an adjacent area:

Evapotranspiration was also linearly (r = 0.87) related to cumulative evaporation from a Class A pan placed on an elevated platform at crop canopy level (4.57 m). In this case the corresponding relationship was:
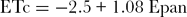
In this location, the seasonal (annual) evapotranspiration totalled about 2200 mm. Cumulative relationships like these always need to be viewed with caution.
In the islands of Guadaloupe (16°N) and Martinique (14°N), six drainage lysimeters (2 × 2 m square × 1.5 m deep; single plants) were used to measure actual rates of water use over a 16 month period (1974/5). Peak rates of evapotranspiration (8–10 mm d−1) were up to 1.6 times the calculated potential rates from a grass reference crop (Penman equation), or 1.4 times evaporation from a USWB Class A pan (Meyer and Schoch, Reference Meyer and Schoch1976).
In Darwin, Australia (12.4°S alt. 0 m), Lu et al. (Reference Lu, Woo and Liu2002) used the sap-flow technique to measure the diurnal water use of whole-plant, pot grown and field planted banana (cv. ‘Williams’ AAA Cavendish subgroup) during the dry season. ‘Granier’ sensor probes were inserted in the upper region (above ground) of the central cylinder of the rhizome. Diurnal rates of water use were positively and linearly correlated with solar radiation (range 0–1.0 kW m−2) and saturation deficit of the air (0–5 kPa). The daily water use of 2.5 m tall (11 leaves, 3.8 m2 total leaf area) field grown plants was 9–10 l (equivalent to only 2 or 3 mm d−1 at plant densities of 2000 or 3000 ha−1 respectively), substantially less than the gross irrigation rate (42 l d−1) then recommended for the Darwin region. The low sap flux densities recorded were attributed to the small leaf area/sapwood area ratio relative to those of other ‘woody’ species.
In semi-arid northeastern Brazil (9°9′S alt. 365 m), Bassoi et al. (Reference Bassoi, Teixeira, Filho, Moura e Silva, Gomes da Silva, Ramos and Sediyama2004b) monitored crop water use over a 33-month period (from planting in 1999 to the end of the third harvest in 2001) for cv. ‘Pacovan’ (AAB Prata subgroup). The soil was a low water holding latosol and the crop was irrigated with micro-sprinklers at Ψm = −30 kPa as recorded at 0.4 m depth by tensiometers. The total surface area between plants, spaced 3 × 3 m, was wetted. Actual crop water use (ETc), excluding drainage, was determined using the water balance approach, and related to reference crop evapotranspiration (ETo) as estimated by a USWB Class A pan (Doorenbos and Pruitt, Reference Doorenbos and Pruitt1977) and the FAO Penman-Monteith (P-M) method (Allen et al., Reference Allen, Pereira, Raes and Smith1998) to develop crop coefficients (Kc).
Values of Kc obtained for i) the vegetative growth stage (from planting to the start of flowering, 211 d) were 0.7 ± 0.3 (pan), or 0.8 ± 0.3 (P-M), followed by ii) first flowering (121 d), 0.9 ± 0.3 (pan) and 1.1 ± 0.4 (P-M), and iii) from first harvest (plant crop) to flowering of first ratoon (single sucker), 110 d, 1.0 ± 0.5 (pan) and 1.1 ± 0.5 (P-M). Values then declined iv) to 0.8 ± 0.4 (pan) and 1.0 ± 0.4 (P-M) from then until the start of the flowering of the second ratoon (217 d), and afterwards v) up to and during the third harvest (with no suckers present) to 0.7 ± 0.4 (pan) and 0.8 ± 0.5 (P-M). Note that the standard errors presented are suspiciously large, and that the crop factors associated with the pan estimates of ETo are always greater than the Penman-Monteith values.
Recently, Montenegro et al. (Reference Montenegro, Gomes, Rodrigues de Miranda and Crisostomo2008) have reported the results of a similar study undertaken in a coastal region of Brazil (3° 28′S alt. 31 m). Actual water use (ETc) was measured over two production seasons (2004–2005, 680 d) using the water balance approach (based on tensiometers) for an irrigated crop (microsprinklers; cv. ‘Pacovan’ AAB Prata subgroup; double row spacing 4.0 × 2.0 × 2.4 m). These values were then compared with Penman-Monteith estimates of reference crop evapotranspiration (ETo) for different growth stages to obtain the corresponding crop coefficients (Kc). Average ETc values increased from 2.6 mm d−1 for the initial vegetative stage of the plant crop up to 4.3 mm d−1 for the flowering and fruit development stage for the ratoon crop. The corresponding average Kc values were 0.60 (0–170 d), 1.05 (plant crop, flowering and fruiting, 240 – 360 d) 0.86 (ratoon crop, vegetative, 415–560 d) and 1.05 (580–680 d). Although no standard errors are presented, these are clear and convincing estimates of both ETc and Kc for an irrigated crop in this location.
On the coastal plain in Surinam (5° 47′N alt. 14 m), Van Vosselen et al. (Reference Van Vosselen, Verplancke and Van Ranst2005) made a brave, but largely unsuccessful, attempt to calibrate and validate a model (SWAP) to assess the water requirements of banana. It was difficult to specify precisely enough the boundary conditions, especially those associated with a high water table and a swelling clay soil. The availability of reliable data with which to run the model was also a constraint compared with a conventional water balance approach.
Subtropics
Following the detailed studies by Robinson and Bower (Reference Robinson and Bower1988) of transpiration from individual leaves of well-watered plants, Robinson and Alberts (Reference Robinson and Alberts1989) reported the seasonal variations in the crop coefficient (ETc/Epan, where Epan is evaporation from a USWB Class A pan) for cv. ‘Williams’ (AAA Cavendish subgroup), planted at a density of 1666 ha−1. Soil samples were taken from positions midway between two plants, at 0.1 m depth increments down to 0.5 m, and the water contents were determined by drying to a constant weight. These values were converted to the corresponding volumetric water contents using the appropriate dry bulk density value. The soil was a sandy clay loam (density 1.68 g cm−3) overlying a clay loam (1.60 g cm−3). Samples were taken the morning following irrigation (by micro-sprinklers), and again immediately prior to the next irrigation at an adjacent point. Estimates of water loss were made in the four main seasons for the second ratoon crop, and only in the summer for the third ratoon, in selected treatments within an irrigation experiment. There were five replicate samples at each point.
Despite all these precautions variability between replicates was large (coefficient of variation 44%). The authors therefore recommended that the data should be treated with caution. In the spring and autumn ETc/Epan ratios were similar at about 0.6–0.7. In the summer the ratio increased to about 1.0, but was only 0.6 in the winter. Evapotranspiration rates in the summer reached 7.3 mm d−1, but only 3.5 mm d−1 in the winter. Most (67–80%) of the water was extracted from the surface down to 0.3 m depth only across all treatments, mainly from the 0–0.1 m layer (up to 48%). Some water (ca. 15%) came from the depth increment 0.4–0.5 m in the drier treatments in the summer months.
In the subtropics of Australia and South Africa plants remain functional throughout the year, although low temperatures in the winter restrict growth rates. The seasonal variation in the ETc/Epan ratio observed in these studies by Robinson and Alberts (Reference Robinson and Alberts1989) confirms the findings of Robinson and Bower (Reference Robinson and Bower1988) summarized above. Namely, that the transpiration rates from a banana plantation in the subtropics are not a fixed function of evaporation from an open water surface. Robinson and his co-authors explain this on the basis of the controlling influence of low soil temperatures on root activity during the year which influences seasonal water use. In the winter months this is independent of the leaf area index. They concluded with the recommendation that ‘evaporation pans and crop coefficients should be used with caution in the subtropics’. Data presented by Turner (Reference Turner1987) suggest that very little water is used by bananas during the winter in northeastern New South Wales, Australia. This is despite large areas of leaves on the plants and suggests increased resistance to water flow through the soil/plant system. These observations are consistent with the work in South Africa.
In the Canary Islands (28° 22′N alt. 295 m), Santana et al. (Reference Santana, Suarez, Fereres and Lopez-Galvez1993) determined the water use of drip irrigated banana (AAA Cavendish subgroup), and the associated crop coefficients (Kc), using two 60 m3 drainage lysimeters (10 plants each). Over a 360-day period, ETc rates varied from 1.5 to 4.6 mm d−1 (averaged over 10 day intervals), depending on the season, with an annual ETc total of 1127 mm. Over the same time periods, Kc values ranged between 0.50 and 1.30 (ETc/Epan screened USWB Class A), and from 0.48 to 1.69 (ETc/ETo Penman-Monteith), with the minimum values in the spring (May). There were very highly significant linear relations between Kc and the proportion of ground shaded by the canopy, as recorded at solar noon.
Mediterranean climates
In Mediterranean climates, the leaves of banana die back in the winter months, explaining the low ETc/Epan ratios at this time (Lahav and Kalmar Reference Lahav and Kalmar1988). At Tyr in the south of Lebanon (33°16′N), a large drainage lysimeter (7 × 7 m square × 1.2 m depth of soil) was used to measure the actual water use of five plants (plant crop) spaced 3 m apart in a triangular array, over a 20-month period through 1971 and 1972. At this high latitude location, evapotranspiration rates during the winter months averaged only 1–2 mm d−1 increasing through the spring and early summer before peaking in July and August at 5 mm d−1 in the plant crop, and 6 mm d−1 in the first ratoon, and then declining rapidly through the autumn. During the period covered, the Kc factor for a USWB Class A evaporation pan ranged, on a monthly basis, from 0.41 after planting to a peak of 1.13 late in the first ratoon. Over the 12-month, first ratoon, period Kc averaged 0.78, and 0.82 for the six months (May–October) when irrigation was applied. When compared with the Penman Eo (open water) estimate the corresponding Kc values were 0.90 and 0.85 respectively. Water was extracted from the soil to depths of 0.6–0.8 m, by plants both within and outside the lysimeter (Bovee, Reference Bovee1975).
Later, Israeli and Namiri (Reference Israeli and Nameri1987) used nine drainage lysimeters (about 1.2 m deep and 4.5 m3 soil volume) to measure the water use of the banana (cv. ‘Williams’ AAA Cavendish subgroup) over a period of six years (1978–83) in the Jordan Valley of Israel (ca. 32°N alt. −210 m). The plants were irrigated through a drip system and drainage water was collected every 10 d. Seasonal water use for the ratoon crops increased from about 1.5 mm d−1 in April, at the start of the season, to peaks of about 7.9 mm d−1 in July and August before declining to 2 mm d−1 in November. A regression between water-use (ETc; mm d−1) and evaporation from a USWB Class A pan (Epan; mm d−1) and the average leaf area (L; m2) accounted for 92% of the variation over the 39 months of measurements (n = 39):
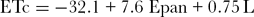
Normalizing for leaf area (to the power 2/3) resulted in the following linear relationship (r 2 = 88%):
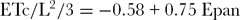
When an additional allowance was made for the age of the plants, there was a small improvement in the precision of this estimate (r 2 = 92%).
In a short-term (one month) study Liu et al. (Reference Liu, Cohen, Tanny, Lemcoff and Huang2008b) compared measured transpiration rates of well-watered bananas grown in a greenhouse in Israel in the winter with estimates of ETo calculated using a number of models, including the FAO Penman and FAO Penman-Monteith equations (Allen et al., Reference Allen, Pereira, Raes and Smith1998), and a standard Chinese 200 mm diameter 110 mm deep evaporation pan. Linear relations were derived between daily transpiration and ETo for each method, with the pan method giving the best agreement (ß = 0.82, r 2 = 83%, n = 21).
Following the research by Lu et al. (Reference Lu, Woo and Liu2002) in Darwin (described above), Liu et al., (Reference Liu, Cohen, Tanny, Lemcoff and Huang2008a) used the same sap flow method to estimate the transpiration of pot-grown banana plants in a greenhouse in Israel (32°0′N alt. 50 m) in winter months. When the effective radius for sap flow in the rhizome was assumed to be 0.63R, rather than 0.60R (where R is the radius of the rhizome), there was a linear relationship (ß = 0.90, r 2 = 79%, n = 16) between daily sap flow estimates and the corresponding gravimetric measurements of transpiration. There was evidence that sap flow lagged 45 minutes behind transpiration for four hours early in the morning, equivalent to 10.5% of daily transpiration, with gradual recovery in the afternoon. Actual daily water use averaged 1.46 l plant−1, over the 16 days of measurement, substantially below the values reported by Lu et al. (Reference Lu, Woo and Liu2002) in northern Australia, due to the corresponding low radiation intensities in Israel in the winter.
FAO reconciliation
In an attempt to reconcile conflicting evidence and to produce standardized procedures for estimating the water requirements of the banana worldwide, Doorenbos and Kassam (Reference Doorenbos and Kassam1979) recommended the following values of the crop coefficient (Kc) based on the relationship given below:
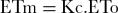
where ETm is the maximum rate of evapotranspiration from a banana crop, ETo is the potential evapotranspiration from a reference crop, short grass or alfalfa, calculated using one of four methods proposed by Doorenbos and Pruitt (Reference Doorenbos and Pruitt1977).
For a plant crop (first year) in the humid subtropics, Kc values ranged from 0.55 up to 1.0 depending on the stage of growth. In the dry subtropics with strong winds, they ranged from 0.45 up to a peak of 1.2. For the first ratoon (second year) the corresponding values were from 0.7 to 1.05, and from 0.7 to 1.25. For a tropical climate, Kc values increased from 0.4 in the first month after planting to 1.05 after 15 months.
In the subsequent FAO manual on crop evapotranspiration (Allen et al., Reference Allen, Pereira, Raes and Smith1998), the tabulated Kc values for a plant crop (maximum height 3.0 m) ranged from 0.50 (early season), to 1.10 (mid season), to 1.00 (end of season). The corresponding values given for a first ratoon crop (4.0 m tall) were 1.00, 1.20 and 1.10. These values are for well-managed crops grown in a sub-humid climate (minimum relative humidity ca. 45%). If, instead of a single crop coefficient, Kc is derived from its two constituent components, transpiration and bare soil evaporation, the corresponding values are given as 0.15, 1.05 and 0.90 (year 1) and 0.60, 1.10 and 1.05 (year 2), assuming a dry soil surface. In all these cases, the FAO version of the Penman–Monteith equation must be used to estimate ETo. The validity of these Kc values, which appear to be realistic, remains to be confirmed.
Conclusions
In the tropics
• Stem flow can account for 10% of incident rainfall.
• Lysimeter studies have indicated that cumulative ETc is linearly related to cumulative evaporation from a conventionally sited USWB Class A pan (Epan) with slopes of 1.2–1.4 and peak rates of water use as high as 8–10 mm d−1.
• Sap flow measurements by contrast suggest transpiration rates as low as 2–3 mm d−1, a suspiciously low value.
• Water balance studies have identified Kc values for different growth stages for the plant crop and the first ratoon. These range from 0.6 to 0.7ETo (vegetative), and 1.0 to 1.1ETo (flowering/fruit development), with actual ETc rates reaching 4.3 mm d−1.
In the subtropics
• Transpiration rates from a banana plantation in the subtropics are not a fixed function of evaporation from an open water surface. As a result, there are seasonal differences in Kc values ranging from 0.5 to 0.6 Epan in the winter months to about 1.0 Epan (or above) in the summer. The corresponding ETc rates increase from 3.5 to 7.3 mm d−1 (based on a water balance approach). Caution is urged when using evaporation pans for scheduling irrigation.
In Mediterranean climates
• In these locations, leaves of the banana also die back in the winter. ETc rates vary from 1–2 mm d−1 in the winter up to 5–8 mm d−1 in the summer. The corresponding Kc values range from 0.4 to 1.1 Epan (using lysimeters).
YIELD RESPONSES TO IRRIGATION
The quality of the papers reporting the results of irrigation experiments designed to quantify yield responses to water is very variable. Emphasis here is placed on those that provided information of more than local interest. Far too many experiments generate data that are site and time specific.
Tropics
Ghavami (Reference Ghavami1974) reported the results of an irrigation experiment conducted in the Sula Valley, Honduras (ca. 15°20′N alt. 30m) over a three-year period (1968–1971) with cv. ‘Valery’ (AAA Cavendish subgroup). Variable amounts of water were applied through under-tree sprinklers (from 25 to 83 mm weekly, inclusive of rainfall (average annual total 1140 mm), or half these quantities twice a week), but independent of evaporation rates. There was no unirrigated control treatment. They concluded from an analysis using third order polynomial equations that a gross weekly water application need not exceed 44 mm, and that there were no benefits from irrigating more often than once a week. Yields of fresh fruit averaged across treatments were 55 t ha−1.
The results of an experiment in St Lucia (14°N) on the effects of irrigation, at different levels of depletion of the available soil water, on the growth and yield in the plant and first ratoon crops (cv. ‘Robusta’ AAA Cavendish subgroup) were reported by Holder and Gumbs (Reference Holder and Gumbs1983a). The paper did not describe exactly how the water regimes were determined or how much water was applied, but harvested yields (see below for definition), 40 weeks after planting, were increased by 13 to 17% (from about 28 to 33 t ha−1) with irrigation. The largest benefits were achieved in the most frequently irrigated treatments (soil returned to field capacity at 25 or 33% depletion of the available water). This followed an apparent increase in the proportion of harvested plants, from 82 to 91%, and a reduction in the number of broken pseudostems (from 10 to 0.9%).
For the first ratoon crop the irrigation treatments were modified, with either 50% replacement of the soil water deficit at eight or four day intervals, or 100% replacement at two day intervals. The potential yield, defined as the product of the actual fresh weight of bunches with fruits within the specified size grade (23–32 mm) and the plant density, was increased from 46 (unirrigated) to 54 t ha−1 (wettest treatment). By contrast, the harvested yields, defined as the product of the potential yield and the proportion of harvested bunches 70–73 weeks after planting, were reduced from 38 to 35 t ha−1 by frequent irrigation. This time, irrigation reduced the proportion of harvested bunches (from 82 to 65%), and increased the number of broken pseudostems (from 16 to 31%) due to extra wind damage.
In the plant crop, irrigation had no effect on any of the vegetative characteristics recorded before bunch emergence, but there was a small increase (ca. 1) in the number of leaves at harvest. In the first ratoon crop, irrigation increased the height and diameter of the pseudostem, but not the number of leaves at harvest. Irrigation advanced the time from planting to shooting by up to three weeks, and the time to harvest by 24 days.
In the plant crop, irrigation had no effect on the numbers of hands per bunch (7–8), but there was a small increase in the numbers of fingers per bunch (from 127 to 131) and in the fresh bunch weight (from 20 to 21 kg). In the ratoon crop, each of the components of yield was increased by frequent irrigation; the number of hands per bunch from 9 to 10, fingers per bunch from 161 to 192, and bunch weight from 27 to 31 kg. It is difficult to draw clear conclusions on whether irrigation is worthwhile from this report.
Holder and Gumbs (Reference Holder and Gumbs1983b) also attempted to compare how two cultivars of the Cavendish sub-group responded to irrigation, ‘Robusta’ (AAA), which dominates trade in the Windward Islands, and ‘Giant Cavendish’ (AAA), which is considered to be susceptible to drought. ‘Partial’ (50% soil water replacement at 4 and 8 d intervals) was compared with ‘full’ irrigation (every 2 d) and an unirrigated control in the ‘plant’ and the two following ratoon crops in a factorial experiment on a clay loam soil in St Lucia. No data on the depths of water applied are presented, nor indeed on the yield responses to irrigation as such. ‘Giant Cavendish’, the shorter of the two cultivars, outyielded ‘Robusta’ (by 13%) over the three cropping cycles. Irrigation increased the susceptibility to wind damage, especially of ‘Robusta’. There were no differences in fruit yield per plant, pulp and peel consistency and bunch uniformity between the two cultivars. ‘Giant Cavendish’ was more susceptible to bunch deformities such as ‘choking’ and ‘openhandedness’ when droughted, but despite this the authors supported its suitability for rain-fed and irrigated production in the Caribbean. The responses of the same two cultivars, with and without irrigation, to three (large) levels of nitrogen fertilizer (280, 560 and 840 kg N ha−1) recorded in the same experiment have also been reported (Holder and Gumbs, Reference Holder and Gumbs1983c). Most yield, and other, differences were small and insignificant. Wind damage restricted any commercial benefits.
Madramootoo and Jutras (Reference Madramootoo and Jutras1984) reported the use of drip irrigation on a heavy montmorillonitic clay soil again in St Lucia in the eastern Caribbean (14°N). Supplementary watering was applied to the plant and first ratoon crops during the relatively dry, or less wet, period from January to May. The crop and the irrigation system were both managed by the farmer on 0.5 ha of land. Water was applied on a daily basis to the irrigated plots whenever rainfall was less than 5 mm, the assumed daily rate of evapotranspiration. In the two years, 635 and 720 mm of water were applied. Irrigation resulted in a small yield increase (7%) in the plant crop, on a base yield of 34 t ha−1, and a small yield reduction in the ratoon crop, due it is claimed to water logging and a high water table. In the second ratoon, a hurricane severely damaged the crop. It was difficult to manage the irrigation system on this poorly draining soil.
In Bangalore, India (13°58′alt. 868 m), Hegde and Srinivas (Reference Hegde and Srinivas1989a) compared the responses of cv. ‘Robusta’ (AAA Cavendish subgroup) to irrigation at four different Ψm values (from −25 to −85 kPa; sandy clay loam soil) as measured at depths of 0.15 m at 0.30 m from the stem. Fruit yields declined from 52 to 41 t ha−1 as the frequency of irrigation decreased. Actual evapotranspiration was measured using a water balance approach and annual totals ranged from 1100 to 1860 mm, giving corresponding water use efficiencies of 37 to 28 kg ha−1 mm−1. Although the experiment ran from 1984 to 1986, it is assumed that these values are annual average responses. Unfortunately, the amounts of irrigation water applied are not recorded. Mid-day leaf water potentials (measured with a Scholander pressure chamber in the pre-flowering period) fell to −0.20 MPa in the wettest treatment, and to −0.62 MPa in the driest. There was some evidence that osmotic adjustment maintained pressure potentials in the leaf. There was no evidence of an interaction between responses to irrigation and to nitrogen fertilizer.
Hegde and Srinivas (Reference Hegde and Srinivas1989b) provided some additional information on the same experiment. Allowing the soil to dry beyond Ψm = −0.45 kPa delayed flowering by up to 30 d and reduced finger and individual bunch weights (from 17 to 13 kg).
Hegde and Srinivas (Reference Hegde and Srinivas1991) later compared the responses of cv. ‘Robusta’ (AAA Cavendish subgroup) to supplementary irrigation, using drip and basin systems, during the plant and first ratoon crops (3086 plants ha−1). Water was applied by the drip system (8 l h−1 single emitter), daily except at weekends, to replace evaporation (0.8 × USWB Class A pan regardless of growth stage) less ‘effective’ rainfall throughout the year. With basin irrigation 30 mm of water was applied into 1.2 m square basins (plants spaced 1.8 m apart) whenever cumulative pan evaporation, minus ‘effective’ rainfall, reached 38 mm. Comparisons of irrigation systems, as such, were therefore confounded with differences in irrigation intervals and amounts of irrigation water applied, which depended on rainfall frequencies and amounts.
There were yield advantages with the drip system in both years (from 73.5 to 83.9 t ha−1 in the plant crop, and from 65.7 to 72.5 t ha−1 in the first ratoon). These followed advancements in the date of flowering, by 14 and 15 d, increases in total dry matter production (13% in both years), and heavier individual bunches (+14 and + 9%) resulting principally from heavier fingers (individual fruits) (+12 and +5%) especially in the plant crop. The efficiency of water use (total yield of fruit, fresh weight, divided by the sum of ‘effective’ rainfall, as defined by the authors, and irrigation water applied) was 13–17% higher with drip than with basin irrigation, from 43 to 49 (plant crop), and from 37 to 43 (first ratoon) kg ha−1 mm−1. About 225 mm more irrigation water was applied with the drip system in both years than with the basin (1470 compared with 1245 mm). There was a corresponding reduction in the depth of ‘effective’ rainfall (from 475 to 275 mm in the plant crop and from 519 to 197 mm in the first ratoon). It is likely that more of the rainfall was ‘effective’ with drip irrigation than with basins, since not all the soil profile was wetted. Using a constant factor (0.8) to convert pan evaporation to ETc was another weakness that reduces the value of this work. Comparing irrigation methods is not easy since many variables can be confounded.
Goenaga et al. (Reference Goenaga, Irizarry and Gonzalez1993) and Goenaga and Irizarry (Reference Goenaga and Irizarry1995; Reference Goenaga and Irizarry1998; Reference Goenaga and Irizarry2000) reported the results of a series of related experiments in the Caribbean island of Puerto Rico. The yield responses of different cultivars to a range of levels of watering based on evaporation from a USWB Class A pan were compared on different soils (mollisol, oxisol and ultisol) in two contrasting locations (18°02′N alt. 21 m; 18°20′N alt. 185 m). One experiment ran for one year only (plant crop, cv. ‘Maricongo’ AAB), and the others for three years with either the plant crop and two ratoons, or three successive ratoons (cvs. ‘Grande Naine’ and ‘Johnson’ both AAA Cavendish subgroup). Water was applied on alternate days through a drip system, and the irrigation treatments were based on pan factors, which increased in 0.25 increments from (variously) 0.0 (rain-fed) to 1.0 or 1.25. Plants were spaced at 1.8 × 1.8 m intervals (overall plant density 1990 ha−1).
The amount of water to apply was calculated as the product of a pan coefficient (kp = 0.7) and a crop coefficient (kc = 0.88), to give an estimate of potential evapotranspiration each week. This was then multiplied by the area of the ‘mat’, and by the appropriate pan factor, from 0.0 to 1.25. Allowance was made for rainfall, and no irrigation was applied if rainfall in the previous week exceeded 19 mm. Fertilizer was either applied in the irrigation water or broadcast. All the yield data were plotted as functions of the pan factor, not the amount of water applied, although these two variables were directly related in individual years. For nearly all the years and sites, there were linear relations between the total bunch yield and the pan factor.
There were similar relationships for individual bunch weights and the number of marketable hands per bunch (sometimes quadratic). Various quality parameters were also often positively related to the pan factor in similar ways. These included: hand weight, fruit length and fruit diameter. Irrigation reduced the number of days to flowering and, to a lesser extent, the number of days from flowering to harvest. The authors concluded that a pan factor of not less than 1.0 should be used when irrigating bananas. This ignores the fact that the response curves to water were nearly always linear throughout the range of irrigation treatments tested. It is a pity that the actual water applications in each year, or evapotranspiration, were not included as the independent variable. Whilst confirming the sensitivity of the banana to water availability, the authors unfortunately made no serious attempt to compare and contrast the results for each cultivar or site so that they could be interpreted and applied with precision to other situations. Some of the results were collated by Goenaga et al. (Reference Goenaga, Irizarry, Coleman and Ortiz1995) to provide practical recommendations for drip irrigation on the semi-arid southern coast of Puerto Rico.
In Hawaii (21° 21′N alt. 6 m), Young et al. (Reference Young, Sammis and Wu1985), developed yield response functions to water using a design which allowed water to be applied, using a drip system, to individual rows at varying rates (from 0.2 to 1.8 Epan in successive increments of 0.2). The volume of water to apply daily to each treatment was calculated using data from a screened USWB Class A pan, adjusted for the ‘mat’ area of individual groups of three plants (cv. ‘Williams’ AAA Cavendish subgroup) spaced at 2.44 × 3.05 m (1343 ha−1). When rainfall was equal to or exceeded 38 mm in the previous week no irrigation water was applied in the following week to any of the treatments. Yearly totals of evapotranspiration were calculated using a water balance approach. When rainfall came in light showers it was assumed that there was no deep drainage, but if more than 38 mm fell in a week drainage followed. Changes in soil water content from one year to the next in the shallow root zone were assumed to be small (maximum 100 mm) compared with changes in other components of the water balance. The soil was kaolinite clay with weathered gravel.
The fruits were harvested weekly from ratoon crops for a period of two years. Since it took about 12 months for each sucker to develop and to produce fruit, evapotranspiration totals were calculated, for each treatment, for successive 52-week periods beginning 12 months before yields were recorded. This corresponded, approximately, to the period of production of each fruit bunch. In the first year the rainfall totalled 860 mm and in the second year 1390 mm; the corresponding estimates of deep drainage were 220 and 731 mm. Yields of fresh fruit (Y, t ha−1) were linearly related to the estimated evapotranspiration total (ETc, mm) during the previous 52 weeks. The slopes and the intercepts of the lines varied in each year.
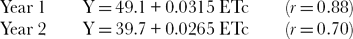
In both cases, the driest treatment (0.2 Epan) was excluded from the analysis (because there were no guard rows) and the results of one treatment from an adjacent experiment added (n = 9).
Since the intercept on the yield axis is positive and large, the relationships are clearly limited to the ETc range from which they were developed (about 1100 to 2700 mm, similar in both years). The corresponding annual yields (actual) were large and ranged from 67.5 to 131 t ha−1.
Following Doorenbos and Kassam (Reference Doorenbos and Kassam1979), see below, a single relationship was developed for both years relating the ‘relative yield loss’ (1 − Ya/Ym, where Ya is the actual yield and Ym is the maximum yield recorded in each experiment) to the so-called ‘evapotranspiration deficit’ (1 − ETa/ETm, where ETa and ETm represent the actual evapotranspiration totals corresponding to Ya, for each treatment, and Ym respectively). Thus:
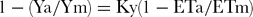
The slope of this linear relationship is known as the ‘yield response factor’ (Ky) for which Young et al. (Reference Young, Sammis and Wu1985) calculated a value of 0.63 (r = 0.77; n = 18). This compares with the range of values proposed by Doorenbos and Kassam (Reference Doorenbos and Kassam1979) of 1.2 to 1.35, for crops yielding 40–60 t ha−1. Values of Ky less than 1.0 indicate relative insensitivity of yield to water deficit, and values above 1.0 relative sensitivity. Clearly there are big differences in the Ky values reported here and explanations are needed. Unfortunately it is not always obvious from the report by Young et al. (Reference Young, Sammis and Wu1985) how the variables in the water balance were actually calculated and evapotranspiration totals estimated.
In Brazil (9°9′S alt. 365 m), Bassoi et al. (Reference Bassoi, Teixeira, Filho, Moura e Silva, Gomes da Silva, Ramos and Sediyama2004b) related the yield of fresh fruit over three harvesting seasons (totalling 409 t ha−1) to measured crop water use over the same period (964 d, Σ ETa, ca. 3950 mm) to obtain a water use efficiency value of 10.4 kg ha−1 mm−1.
Subtropics
Trochoulias (Reference Trochoulias1973) studied the responses of cv. Williams (AAA Cavendish subgroup) to supplementary under-tree sprinkler irrigation over a three-year period (1968–1970) in New South Wales, Australia (28°51′S alt. 148 m). Allowing the available soil water content to be depleted by 10, 20, 40 or 70% before irrigating the soil (clay loam) back to field capacity resulted in progressively larger reductions in yield. When averaged over all three years, maintaining the soil water content in excess of 90% of the calculated available water capacity, within an assumed root zone of 0.45 m, resulted in the highest yields (ratoon crops). This treatment, which yielded twice as much fruit as the rain-fed, control, involved the application of 8 mm water every 3–5 days when there was no rain. This implies that evaporation rates were only about 1.5–3 mm d−1, values that appear to be low. Total annual water applications were 400–500 mm. Frequent irrigation increased all the components of yield, principally the number of bunches and the number of fingers per bunch.
Later, again in eastern coastal Australia (28° 51′S alt. 148 m), Trochoulias and Murison (Reference Trochoulias and Murison1981) compared different levels of replacement with supplementary drip irrigation (single microtube at each plant station spaced 1.8 m apart) based on evaporation from a USWB Class A pan. Water was applied twice weekly from zero to 1.20 times Epan at 0.20 intervals. If rainfall during each interval exceeded evaporation no irrigation was applied. The experiment continued for six years (1971–1976). The soil was a free-draining clay loam. The treatment effects on fruit yield and its components were small, since four of the six years were ‘very wet’. Nevertheless the authors concluded that drip irrigation was suitable for bananas and that a useful working guide was to apply water at the rate of 0.60 × Epan.
In subtropical northeastern Transvaal in South Africa (23°05′S alt. 750 m), Robinson and Alberts (Reference Robinson and Alberts1987) compared the responses of cv. Williams (AAA Cavendish subgroup), during the first and second ratoons, to under-canopy sprinkler and drip irrigation. Similar amounts of water were applied with both systems, daily in the case of drip (except at weekends!), and every two days with the under-canopy sprinklers in the summer or every 2.5–4 days in the winter. Applications were based on full replacement of the soil water deficit, based on the product of 0.75 × Epan, where Epan is evaporation from a conventionally sited USWB Class A pan, less any rainfall. There were two drippers per plant (spaced 3 × 2 m) each delivering 4 l h−1 in the first ratoon crop, and four drippers per plant in the second ratoon. The sprinklers were spaced at 6 m square with 100% water distribution overlap. This meant that the pseudostems and foliage were wetted to a height of 1.5 m whenever water was applied. Irrigation occurred throughout the year.
There were many interesting findings. Perhaps the most fundamental was that sprinkler irrigation reduced soil (at 0.2 m depth) and pseudostem temperatures by up to 3 °C. It was this effect that probably slowed the rate of emergence of leaves and, surprisingly (?) also increased, by two to three, the number of leaves produced before flower emergence. As a result flowering was delayed in the sprinkler irrigated plants from early summer to the autumn (three to four months), which in turn extended the interval between one harvest and the next, by up to two months, compared with those irrigated by the drip system. In both ratoon crops, there were associated yield advantages with drip irrigation, about 30% per annum (on base yields of 40–50 t ha−1), following the reduction in the duration of the crop cycle and the production of larger bunches (more hands per bunch, more fingers per hand and longer fingers), also linked to the time of the year when flowering occurred, compared with sprinkler irrigated plants.
Assuming that plants in both treatments had similar amounts of ‘available’ water, evaporative cooling appears to have played an important role in differentiating how bananas respond to two contrasting methods of applying water, in an area where pseudostem temperatures in the autumn and winter were close to or below about 22 °C during the daytime. Further analysis of the data showed that a 1 °C reduction in the daily maximum air temperature, over the range 23–32 °C, would reduce the number of leaves produced in a year by 3–4. The effect of a reduction in temperature will however depend on its position on the temperature response curve. For the rate of appearance of new leaves the optimum temperature is near 30 °C (Turner and Lahav, Reference Turner and Lahav1983). We are dealing with complicated but rational systems!
Earlier the same two authors had reported the results of a trial in which the water was applied daily (from Monday to Friday) through a drip irrigation system to cv. Williams (AAA Cavendish subgroup) at the same site in northeastern Transvaal. The soil was a sandy loam overlying a sandy clay loam with a sandy clay below 0.4 m depth. In this subtropical location the annual effective precipitation, falling between October and April, is less than 1000 mm. Robinson and Alberts (Reference Robinson and Alberts1986) compared three different USWB Class A pan coefficients (ETc/Epan) namely 0.25, 0.5 and 0.75. Irrigation was applied throughout the year to supplement rainfall over three cropping cycles, plant crop and two ratoons (1666 plants ha−1). All the plants were irrigated to the same schedule (pan coefficient = 0.25) for the first seven months after planting until the crop cover had reached 40%. Afterwards differential watering was introduced. In the winter months during the second ratoon the three coefficients were reduced by 33% to 0.15, 0.35 and 0.50. Full randomization of the treatments was not possible because of practical constraints with the irrigation equipment. Water was applied at the rate of 4 l h−1, with two emitters per plant (spaced 1 m apart) during the first two years, and four in the third and last year.
Applying insufficient water lengthened the period between planting and the first harvest by about three weeks, and between sucker selection and the harvest of the first ratoon crop, by about six weeks. Applying the highest quantity of water (pan factor = 0.75) increased annual fruit yields by 33, 51 and 8% in the plant, first ratoon and second ratoon crops respectively, compared with the treatment receiving least water (0.25). The second year of the experiment was considered to be an untypical drought year, when excessive evaporation rates linked to high temperatures (> 29 °C) and dry air (> 2.5–3.0 kPa) during part of the season (December to February) contributed to the plant responses observed in the driest treatment. Water deficits also reduced some aspects of vegetative growth including the rate of unfolding of leaves, and the leaf area index at flower emergence (as defined by the authors). The yield benefits recorded in the first ratoon (from 55 to 74 to 83 t ha−1 y−1 from relatively dry to wet, respectively) were associated with an increase in bunch mass (from 32 to 45 kg) resulting from more hands per bunch, more fingers per hand and longer fingers. These benefits were independent of the month of flowering. The total depths of irrigation water applied in that year were 488, 969 and 1453 mm, respectively. These equate to irrigation water use efficiencies of about 40 kg ha−1 mm−1 Similar quantities of water were applied during the second ratoon, a so-called ‘normal year’ in terms of rainfall, but without the same yield differences between the three treatments. The soil water status in all three treatments was similar.
The authors concluded that bananas are sensitive to water deficits at Ψm values as high as −20 kPa (recorded at 0.2 m depth, and 0.2 m from the emitter). They were unable to recommend a standard pan coefficient because of the variability in response between the two years, and therefore supported the use of tensiometers together with an evaporation pan for irrigation scheduling.
Mediterranean climates
In the northern coastal plain of Israel (ca. 33°N), Lahav and Kalmar (Reference Lahav and Kalmar1981) compared the responses of cv. Williams (AAA, Cavendish subgroup), grown on a brown vertisol, to two levels of water application and two frequencies of irrigation over three years (1975–1977). Water quantities were based on evaporation from a USWB Class A pan (times 0.9 during the mid-summer months, but adjusted for leaf area at other times in the growing season) with full (660 mm) or partial (75%, 500 mm) replacement of the estimated soil water deficit. Water was applied, through a drip system (4 l h−1), at intervals of three days, commercial practice at that time, or ‘pulsed’ at hourly intervals over five hours on a daily basis. Fertilizers were injected into the irrigation system at constant rates (30 mg N l−1 and 90 mg K l−1). ‘Pulsing’ with the regular quantity of water always resulted in the highest yield (44 t ha−1 averaged over the plant crop and two ratoons, compared with 41 t ha−1 from the pulsed crop with partial replacement, and 42 and 40 t ha−1 from the two treatments irrigated at three day intervals respectively). The corresponding yield responses to the water applied were equivalent to 66, 82, 64 and 80 kg ha−1 mm−1.
Differences in yield, which were not always consistent between years, were associated with variation in individual bunch weights (averaging 29 kg over three years) and the number of bunches per hectare (1700), associated in part with the effects of the irrigation treatments on the time of flowering. Yield differences between watering treatments were related to the high Ψm values maintained in the frequently irrigated treatments, always above −12 kPa at 0.225 m depth, and to the volume of wetted soil beneath the drippers, which ranged from 44% in the three-day interval treatment, with a reduced quantity of water, 60% for the corresponding ‘pulsed’ treatment, up to about 77 and 72% respectively for the two treatments irrigated with the regular amounts. Pulsing also cooled the soil in mid-summer (by 2–3 °C below 25–26°C, at a depth of 0.1 m, which could be important in areas where temperatures can exceed the optimum), reduced the number of roots in the 1.0 m deep profile by nearly 18%, and reduced nitrate leaching. The authors concluded that shortening the irrigation interval was an effective way of saving water. Applying less water also improved water-use efficiencies.
In experiments lasting five years (1979–1983) in western Galilee in northern Israel, an area of winter rainfall, Lahav and Kalmar (Reference Lahav and Kalmar1988) later studied the responses of Dwarf Cavendish bananas (AAA) to a range of watering regimes using drip irrigation, combined with two fertigation treatments. In this high latitude (ca. 33°N) area, the leaves are killed during the winter but leaf areas increase from March through to August and September before starting to decline. Seasonal irrigation water requirements (evapotranspiration) average about 1100 mm, with peak rates in mid-summer of 6–7 mm d−1. In this trial, on a vertisol soil, there were two lateral pipes per plant row (double rows, 3 × 3 m with 6 m path) with drippers (output 4 l h−1) spaced at 1 m intervals. The irrigation treatments consisted of applying different quantities of water during the season based on variable pan factors and evaporation from a USWB Class A pan. During the mid-summer months (July, August and September) these reached peak values of 0.8, 1.0, 1.3 and 1.4 before declining in proportion. Similarly, values from the beginning of the season in April until July were proportional to the peak values. Irrigation of the control treatment was based on a constant pan factor of 1.0 throughout the season regardless of the stage of growth. Fertilizer was applied in the irrigation water either continuously at a constant concentration or at weekly intervals.
Total water applications varied from 845 mm (0.8 pan factor) to 1447 mm (1.4) averaged over the five years. The corresponding range of nitrogen applications in the continuous treatment was 170–295 kg N ha−1. Irrigation treatment effects were much larger than any influence of fertilizer although weekly applications resulted in small, but non-significant, benefits. Averaged over the five years, irrigating at a pan factor of 0.8 reduced the height of the suckers (by 0.1 m), as measured in the autumn, compared with every other treatment, and also reduced fruit (bunch) yields from 68 to 65 t ha−1. None of the treatments influenced the dates of flowering. This yield difference was attributed to a reduction in the corresponding numbers of bunches, from 1865 to 1775 ha−1, as individual bunch weights were similar at about 32 kg.
The most efficient treatment, in terms of the fresh weight of fruit produced per unit of irrigation water applied, was that in which the least amount of water was applied (factor 0.8) at about 76 kg ha−1 mm−1. The lowest value was 48 kg ha−1 mm−1 (factor 1.4).
Israeli and Nameri (Reference Israeli and Nameri1986) reported the relationships between water use, as determined using drainage lysimeters (Israeli and Nameri, Reference Israeli and Nameri1987), and production, including leaching requirements. These studies were conducted in the Jordan Valley of Israel (ca. 32°N alt. −210 m). There were linear relations between total dry matter production from each ‘mat’ and the actual total water use (evaporation plus transpiration), in each of the three years of the experiment. The slopes of the regression lines were 1.71 (plant crop), 1.60 (first ratoon) and 2.35 g l−1 (second ratoon); the corresponding values for the dry weight of the fruit were 0.78, 0.77 and 0.86 g l−1. The dry weight of fruit was greatest in the first ratoon and least in the plant crop. Since the total plant dry weights were similar in the first and second ratoons the harvest index was greatest in the second year after planting.
FAO reconciliation
Doorenbos and Kassam (Reference Doorenbos and Kassam1979) concluded from their review that the banana requires an ample and frequent supply of water. They quoted annual water requirement totals from 1200 mm in the humid tropics to 2200 mm in the dry tropics. The relationships that they developed from the literature between relative yield loss and relative transpiration deficit, as defined above, were similar for all four growth stages that were rather arbitrarily specified: i) establishment, and early vegetative growth; ii) vegetative when the leaves are developing; iii) flowering, from the start of flower bud differentiation, and iv) yield formation, as the fruits develop. Water deficit during any of these stages was considered to be equally damaging to yield, through effects on either quantity or quality of the fruit. The value of Ky proposed was 1.2–1.35, indicating great sensitivity to water deficit. The irrigation interval, depending on the soil type, rooting depth and evaporation rates would range from as little as three days up to 15 d. They suggested that the allowable soil water deficit should not exceed 35% of the available water in the root zone. Most roots they stated were to be found in the top 0.75 m. of soil. Good commercial yields are in the range 40–60 t ha−1, and water utilization efficiencies (fruit 70% water content) vary from 2.5–4.0 for the plant crop to 3.5–6.0 kg m−3 for the ratoon crops. These values equate to 25–40 and 35–60 kg ha−1 mm−1, which are within the range cited in this text.
Plant density and arrangement
The optimum plant density is difficult to define for specific cultivars and conditions, and there does not seem to have been any research reported which attempts to identify different densities depending on the hydrological regime under which the banana is grown. A universal observation with bananas is the extension of the crop cycle at high densities. Since floral initiation can occur at any time of the year, the harvesting period can, as a result, become similarly extended. Increased competition also leads to greater plant to plant variability and can extend the duration of harvest This may be a result in part of the reduced pseudostem temperature in plants grown at the high density (Robinson and Nel, Reference Robinson and Nel1988; Reference Robinson and Nel1989). Attempts have been made to specify the target leaf area index (L) that will maximize solar radiation interception, production and profitability. Differences in the duration of crop cycles between places and between seasons complicate this approach, and for true comparisons annual yields need to be specified. Using this method, Robinson and Nel (Reference Robinson and Nel1989) identified the optimum density for fruit production for an irrigated crop (cv. ‘Williams’ AAA Cavendish subgroup) in South Africa to be in the range 1800–2000 ha−1 (L = 6) or 1666 ha−1 (L = 5) if other management factors, including the timing of harvests, and cost are taken into account. A further complication is that the optimum density for a plant crop differs from that for a ratoon.
In tropical banana areas, nearly all new plantations are established on a hexagonal system. In the subtropics (South Africa) rectangular, or hedgerow, systems have been preferred because it is easier to identify the rows, but now double rows or ‘tramline systems’ have become popular, particularly in Australia, because these permit easy access by machinery and other practical benefits including irrigation (Robinson et al. Reference Robinson, Nel and Bower1989; Robinson, Reference Robinson and Gowen1995).
Conclusions
It has not always been easy to draw generic conclusions with wide applicability from the irrigation experiments reported. Poor experimental designs together with lack of information and poor/incomplete analysis have limited their value. Rarely have authors considered the weaknesses/limitations in the experimental techniques employed before presenting the results. The need for an integrated approach to irrigation research is highlighted linking empirical field experiments (but well designed and implemented) with supporting environmental physiology measurements, so that the mechanisms responsible for determining the observed yield responses are fully understood, and the results applied elsewhere (time and space) with confidence (Carr, Reference Carr, Ferreira and Jones2000).
In the tropics
• Although there were often, usually small, ancillary benefits from irrigation, including advancements in flowering and harvesting dates and improvements in many aspects of fruit quality (including heavier bunches, more hands per bunch, greater fruit length and diameter), yield increases between sites were variable and inconsistent.
• In Puerto Rico, yields of fresh fruit increased linearly with the quantity of water applied from, for example, 35 to 65 t ha−1 (more in the ratoon crops than the plant crop) based on the range of pan factors tested.
• In Hawaii, annual fresh fruit yields increased linearly as ETc increased by an average of about 30 kg ha−1 mm−1 on base yields of 40–50 t ha−1. This compares with water use efficiencies of 40–50 kg ha−1 mm−1, based on the sum of ‘effective’ rainfall and irrigation, reported in South India, and 10 kg ha−1 mm−1, based on ETc, in Brazil.
• In Hawaii, the corresponding yield response factor (Ky) was 0.63, which is substantially below the range of values (1.2–1.35) proposed by Doorenbos and Kassam (Reference Doorenbos and Kassam1979).
In the subtropics
• To ensure large yields of banana, soil water deficits should be kept low (by maintaining Ψm > −20 kPa at 0.2 m depth). This means irrigation intervals should not exceed 2–3 d during the summer.
• Although annual yield responses to irrigation are variable, water use efficiencies of 40 kg ha−1 mm−1 have been achieved, a value similar to that obtained in the tropics.
• All the components of yield are enhanced by irrigation. Applying insufficient water delays crop development.
• The cooling effect of irrigation with micro-sprinklers on the soil and pseudostem temperatures, compared with drippers, delays crop development and can reduce annual yields by 30%.
• It has not been possible to specify a standard pan coefficient because of variability in yield responses to irrigation between years.
Mediterranean climates
• Using drip irrigation, water use efficiencies of up to 80 kg ha−1 mm−1 (water applied) have been obtained with ‘partial’ replacement (75%) of the soil water deficit, compared with 50–60 kg ha−1 mm−1 with ‘full’ replacement (100%).
• Yield responses are not consistent between years.
Irrigation systems
The choice of irrigation system depends on so many factors that are site and context specific. All can be made to work effectively given appropriate technical skills, financial resources, and awareness. Robinson (Reference Robinson1996) and Daniells (Reference Daniells2004) have reviewed these in the context of banana plantations, whilst Eckstein et al. (Reference Eckstein, Fraser, Botha, Husselmann and Galan1998) reported the preliminary results of a comparison of various irrigation systems at two sites in South Africa. Bananas differ from most other crops in that they are ‘nomadic’. Plant positions change after the plant crop depending on which sucker is selected for the following ratoon crops. In the context of this review, the cooling effects of under-tree micro-sprinklers have to be taken into account when assessing their relative merits. Well-designed and managed micro-sprinklers and drip irrigation systems are likely to be the most efficient and effective methods of applying water to bananas.
GENERAL CONCLUSIONS
With the increasing need to use water effectively, and to maximize water productivity (yield per unit of water consumed) in irrigated agriculture worldwide, there is a continuing need to identify the minimum amount of water need to optimize farm incomes rather than always seeking to aim for maximum marketable yields per unit area. Fereres and Soriano (Reference Fereres and Soriano2006) have recently reviewed the role that so-called ‘deficit irrigation’ (the application of water below ETmax levels) can play in improving the water productivity of field crops, in particular they emphasized how ‘regulated’ deficit irrigation can increase farm profits particularly in fruit trees and vines. With the banana, few experiments have been reported in which the aim was to identify at what stages in the development of the crop, water applications can be reduced below the maximum without a proportional loss in marketable yields (this assumes that there are yield-determining processes that are differentially sensitive to water deficits). As Fereres and Soriano (Reference Fereres and Soriano2006) stated, research linking the physiological basis of these responses (generally well understood for the banana) to the design of practical ‘regulated deficit irrigation strategies’ could have a significant impact in water-limited areas (or where it is expensive to deliver water to the field)Footnote 3. A tall, aerodynamically rough crop like banana is also better coupled to the atmosphere than a short, field crop and a decline in stomatal conductance will be translated into a corresponding reduction in transpiration (and to a large extent photosynthesis). In addition, micro-irrigation systems are ideally suited for controlling water applications and therefore for this form of stress management. Their design and operating criteria, usually the preserve of engineers, need to be specified with appropriate levels of precision (for specific farming systems) in order to maximize (marketable) crop-water productivity, whilst ensuring minimum adverse effects on the water environment (Molden, Reference Molden2007). These are the challenges.
Acknowledgements
The helpful and constructive comments provided by Dr D. W. Turner on this manuscript are gratefully recognized.


