INTRODUCTION
Tibet, as the highest region on the earth with an average elevation of 4000 m, is a plateau region in the northeast of the Himalayas in China. The region is characterized by rarefied air, strong solar radiation, perennial arid environment and low temperatures, and its climate is inherently extreme (Duan & Wu Reference Duan and Wu2005; Liu et al. Reference Liu, Bao, Duan, Qian and Wu2007; Wang et al. Reference Wang, Chen and Qi2009). Most of the local Tibetan people live on raising livestock, such as yaks, cattle, sheep, goats, camels and horses. However, feedstuff shortages due to inherently extreme climates and short growing seasons cause heavy livestock losses (Long et al. Reference Long, Zhang, Wang, Hu and Dong1999; Yu et al. Reference Yu, Zhang, Claus, Zeng, Zhang and Wang2012). Highland barley (Hordeum vulgare L.), which occupies >0.65 of the total food production, is a typical crop well-adapted to the specific geographical environment in the Tibet autonomous region of China. As the primary food for the Tibetan people, highland barley grain has been widely accepted as an important source of brewing materials and a food named tsamba. As an important source of roughage for local animals, highland barley straw (HBS) can to some extent offset the shortage of feedstuffs, especially in the cold season. Until now in China, most studies associated with highland barley have focused on genetic diversity and nutrient accumulation in barley grain, rather than on straw quality. Previous studies have noted that total above-ground biomass of highland barley increased linearly with nitrogen (N) fertilization (120–400 kg N/ha), but excessive N fertilization (>400 kg N/ha) resulted in a reduction in biomass yield (He et al. Reference He, Zhang and Tang2009; Li Reference Li2010; Hu & Yang Reference Hu and Yang2011; Yang Reference Yang2012; Liu et al. Reference Liu, Zhaxi, Zhaxi and Song2013). Knowledge about nutrient accumulation, digestibility and fermentability was not available for HBS as a forage resource in Tibet. Under well-controlled conditions, the objective of the present study was to put forward a suitable urea N fertilization strategy for planting highland barley without compromising the nutrient accumulation, digestibility and fermentation extent of HBS as an important forage resource.
MATERIALS AND METHODS
Experimental site for highland barley plantation
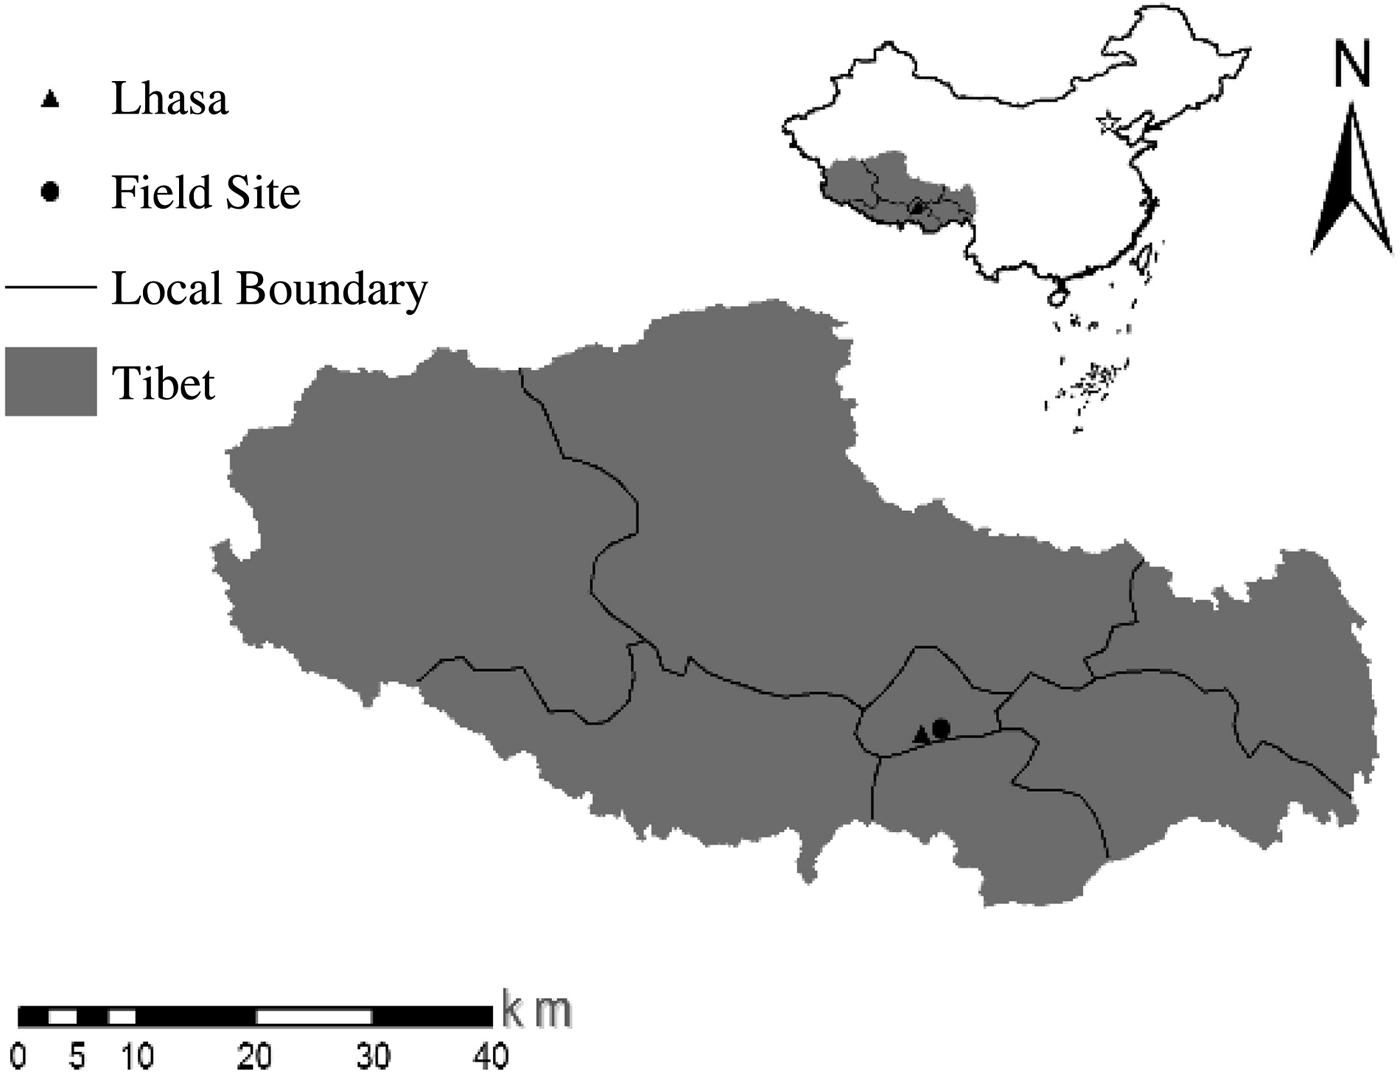
Highland barley (H. vulgare L. Zangqing 320) was planted in the Lhasa Agricultural Experiment Station of the Chinese Academy of Sciences in Tibet on 20 April and harvested on August 2013 when the plant had matured. The site (29°40′ N, 91°20′ E, 3688 m a.s.l., Fig. 1) belongs to the semi-arid temperate plateau monsoon climate zone (Leber et al. Reference Leber, Holawe and Häusler1995). The annual mean precipitation, solar radiation and atmospheric pressure are c. 439 mm, 7026·6 MJ/m2 and 61 k Pa, respectively. Prior to the current experiment, in April 2013, soil samples on the site were collected with a five-spot sampling method. Organic matter content was determined by following the potassium dichromate oxidation method as described by Walkley & Black (Reference Walkley and Black1934). Total nitrogen content was measured with the Kjeldahl method (Bremner & Mulvaney Reference Bremner, Mulvaney and Page1982). Total phosphorous was extracted from soils with 1N HCL after being ashed at 550 °C (Aspila et al. Reference Aspila, Agemian and Chau1976). The field soil was sandy loam and contained 20 g organic matter, 0·84–1·03 g total nitrogen and 0·15–0·26 g total phosphorus per kg air-dried soil.
Experiment site situated in the Lhasa Agricultural Experiment Station, Chinese Academy of Sciences in Tibet at an altitude of 3688 m.

Experimental design and highland barley straw harvest
A completely randomized design of planting highland barley in 36 field plots (3 × 5 m) at the experimental site was applied to investigate the effect of different urea fertilization levels on biomass yield and nutritive quality of highland barley. Six urea N levels of 0 (control), 156, 258, 363, 465 and 570 kg/ha were applied. Each urea N amount was divided into three portions (e.g. 0·4, 0·3 and 0·3 of total amount), and evenly spread onto the soil surface prior to irrigation at seeding (growth stage (GS) 0), stem elongation (GS 32) and heading (GS 49), respectively. The definition of each GS was referred to the method as described by Zadoks et al. (Reference Zadoks, Chang and Konzak1974), in which for example, GS 0 represents the dry seed stage (day 1); GS 32 represents the growth day when the second node can be observed (day 53–55); GS 49 represents the time first awns visible (day 64–69). Six field plots were arranged for each fertilization level treatment in the present study.
During planting, highland barley seeds were drilled with 25 cm spacing between rows. Day of maturity was determined according to the hardness of the kernels (i.e. how easily they could be scratched with the thumbnail) and stem diameter was measured at the middle of the first internode. After the plant height was measured, the plants within each plot were harvested 3–4 cm above ground level, the highland barley grains removed and 36 HBS samples (500 g) obtained. Every HBS sample was divided into two portions: one was reserved for chemical analysis and the other used to measure leaf and stem components. During harvest, the whole plant, grains, HBS, leaf and stem materials were weighed individually. To determine the dry matter (DM) yield, all plant samples were oven dried at 65 °C until a constant weight was observed. The HBS samples obtained from all field plots were ground in a ball mill, passed through a 1 mm screen and stored at –4 °C for later chemical analysis and in vitro batch cultures.
Rumen fluid collection
Rumen fluid collection and in vitro batch cultures were performed at the State Key Laboratory of Animal Nutrition of China Agricultural University. Four rumen-cannulated lactating Holstein dairy cows (body weight = 530 ± 31 kg; days in milk = 51 ±8 days; daily milk yield = 17·2 ± 0·77 kg) were used as donor animals for rumen fluid collection. The animals were housed in individual tie stalls (9 m2), each with separate water and feed bunk. The cows’ daily feed was 4·0 kg alfalfa hay, 3·5 kg whole maize silage and 5·5 kg commercial concentrate consisting of 530 g maize meal/kg, 140 g soybean meal/kg, 70 g cotton seed meal/kg, 40 g rape seed meal/kg, 120 g distillers dried grains/kg, 10 g limestone/kg, 10 g calcium hydrogen phosphate (CaHPO4)/kg, 10 g sodium chloride (NaCl)/kg, 10 g sodium bicarbonate/kg and 10 g trace mineral/kg and vitamin premix. The ration was divided equally into two portions and fed at 07 : 00 and 19 : 00 h, respectively. Rumen fluid, obtained from four animals 1 h before the morning feeding, was filtered through four layers of gauze and mixed in equal proportions to achieve a representative rumen fluid, held in a water-bath at 39 °C in an atmosphere of carbon dioxide (CO2) and used in the later in vitro batch culture. All animal care, surgical procedures, and rumen fluid collection were approved by the Institutional Animal Care and Use Committee at China Agricultural University.
In vitro batch culture and sampling procedure
Highland Barley straw samples (500 mg each) were weighed into a total of 72 glass bottles (six urea N levels × six field plots × two bottles per plot) with butyl rubber stoppers. Fresh buffer solution (pH 6·8) was prepared following the method of Menke & Steingass (Reference Menke and Steingass1988). Under a stream of nitrogen gas (N2), each bottle was inoculated with 50 ml of the buffer solution followed by 25 ml of filtered rumen fluids. Afterwards, each bottle was purged with anaerobic N2 for 5 s to remove headspace air, sealed with a butyl rubber stopper and a screw cap. Thirty six bottles were individually connected with medical plastic infusion pipes to gas inlets of an automated trace gas recording instrument (AGRS-III, China Agricultural University, Beijing, China) to continuously record the gas production (Zhang & Yang Reference Zhang and Yang2011). Three fermentations without the substrate were included as blanks. Meanwhile, another 36 bottles were purged with anaerobic N2 for 5 s, sealed with butyl rubber stoppers and individually connected to emptied air bags to collect the fermentation gases for later analysis of CO2, methane (CH4) and hydrogen gas (H2); three fermentations without a substrate were also included as blanks. All bottles were incubated at 39 °C for 72 h. The batch cultures were repeated in three experimental runs.
After each run of 72 h incubation, the cumulative gas production volumes against incubation time were exported into a Microsoft Excel datasheet from the AGRS-III and three 1·0 ml gas samples were taken by syringe from the air bags for later analysis. The entire biomass cultures (75 ml) in all bottles were transferred to falcon tubes (100 ml) and centrifuged at 3500 g at room temperature for 15 min. The final pH of the supernatant was measured immediately using a pH meter. A first aliquot of the supernatant (5 ml) was transferred to a polypropylene tube for microbial N analysis. A second aliquot (5 ml) was transferred to a polypropylene tube containing 0·5 ml of 50 g H3PO4/l for ammonia N analysis. The third aliquot (1 ml) was transferred to a polypropylene microtube containing 0·3 ml of 250 g orthophosphoric acid/l solution, and the mixture was cooled at 4 °C for 2 h and centrifuged at 15 000 g for 10 min at 4 °C. Finally the supernatant was frozen at –20 °C for volatile fatty acid (VFA) analysis.
Chemical analysis
The chemical composition of the HBS samples were analysed following the AOAC methods for DM (ID 930·5), ether extract (ID 920·30) and ash (ID 942·05) (AOAC 1999). The chemical composition of the leaf and stem samples were analysed following the AOAC (1999) method for crude protein (CP, ID 984·13). Both neutral detergent fibre (NDF) and acid detergent fibre (ADF) corrected for residual ash content were measured following the methods of Van Soest et al. (Reference Van Soest, Robertson and Lewis1991).
Microbial N concentration in culture fluids were determined based on purines using the method of Zinn & Owens (Reference Zinn and Owens1986) as modified by Makkar & Becker (Reference Makkar and Becker1999). Ammonia N concentration was measured following a spectrophotometric method as described as Verdouw et al. (Reference Verdouw, Van Echteld and Dekkers1978). The concentrations of acetate, propionate, butyrate, valerate, iso-butyrate and iso-valerate in the supernatants of the culture fluids, and CH4, CO2 and H2 in the fermentation gas samples were measured by a gas chromatograph (GC522, Wufeng Instrument, Shanghai, China) following the methods of Zhang & Yang (Reference Zhang and Yang2011).
Biometric analysis
The cumulative gas production (GP t, ml/g DM) at time (t) was fitted to an exponential model (Eqn (1)) by iterative regression analysis (France et al. Reference France, Dijkstra, Dhanoa, Lopez and Bannink2000) using the nonlinear procedure of the software package SAS for Windows (version 9·02; SAS inst., Cary, NC, USA):
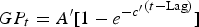 $$G{P_t} = A^{\prime}[1 - {e^{ - c^{\prime}}}^{(t - {\rm Lag})} ]$$
where A represents the asymptotic GP generated at a constant fractional rate (c) per unit time (h); e is the base of a logarithm; t is the gas recording time (h), and Lag stands for a lag time phase (h) before the GP commenced.
Following the method of García-Martínez et al. (Reference García-Martínez, Ranilla, Tejido and Carro2005), the average gas production rate (AGPR, ml/h) between the start of the incubation and the time at which the cumulative gas production was half of its asymptotic value was calculated as:
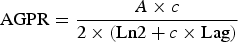 $${\rm AGPR} = \displaystyle{{A \times c} \over {2 \times ({\rm Ln}2 + c \times {\rm Lag})}}$$
The sum of the analysed CH4, CO2 and H2 was calculated as the total gas produced in molar proportion (mol/100 mol), which excluded N2, residual O2 and water vapour in the head space gas of each bottle. Finally, molar proportions of CH4, CO2 and H2 in total fermentation gases were calculated prior to statistical analysis. Branched-chain VFA (BCVFA) was calculated as a sum of iso-butyrate and iso-valerate. The ratio of non-glucogenic to glucogenic acids (NGR) was calculated (Ørskov Reference Ørskov1975) as:
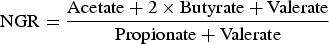 $${\rm NGR} = \displaystyle{{{\rm Acetate} + 2 \times {\rm Butyrate} + {\rm Valerate}} \over {{\rm Propionate} + {\rm Valerate}}}$$
Based on chemical analysis and gas production, metabolizable energy (ME) values were calculated following the equations recommended by Close & Menke (Reference Close and Menke1980) and Menke & Steingass (Reference Menke and Steingass1988).
One-way analysis of variance of data was performed using the general linear model procedure of the software package SAS for Windows (version 9·02; SAS inst., Cary, NC, USA). Urea N level was included as fixed effect in the model. Least square means and standard error (s.e.m.) were calculated using the least square means procedure of the SAS software package, and orthogonal polynomial contrasts were performed to determine linear and quadratic effects of the urea N fertilization within the urea N fertilization levels. Correlation coefficients between chemical composition and fermentation characteristics were calculated using the SAS software package. Significance was declared at P < 0·05.
RESULTS
Effect of urea nitrogen fertilization on highland barley growth and biomass yield
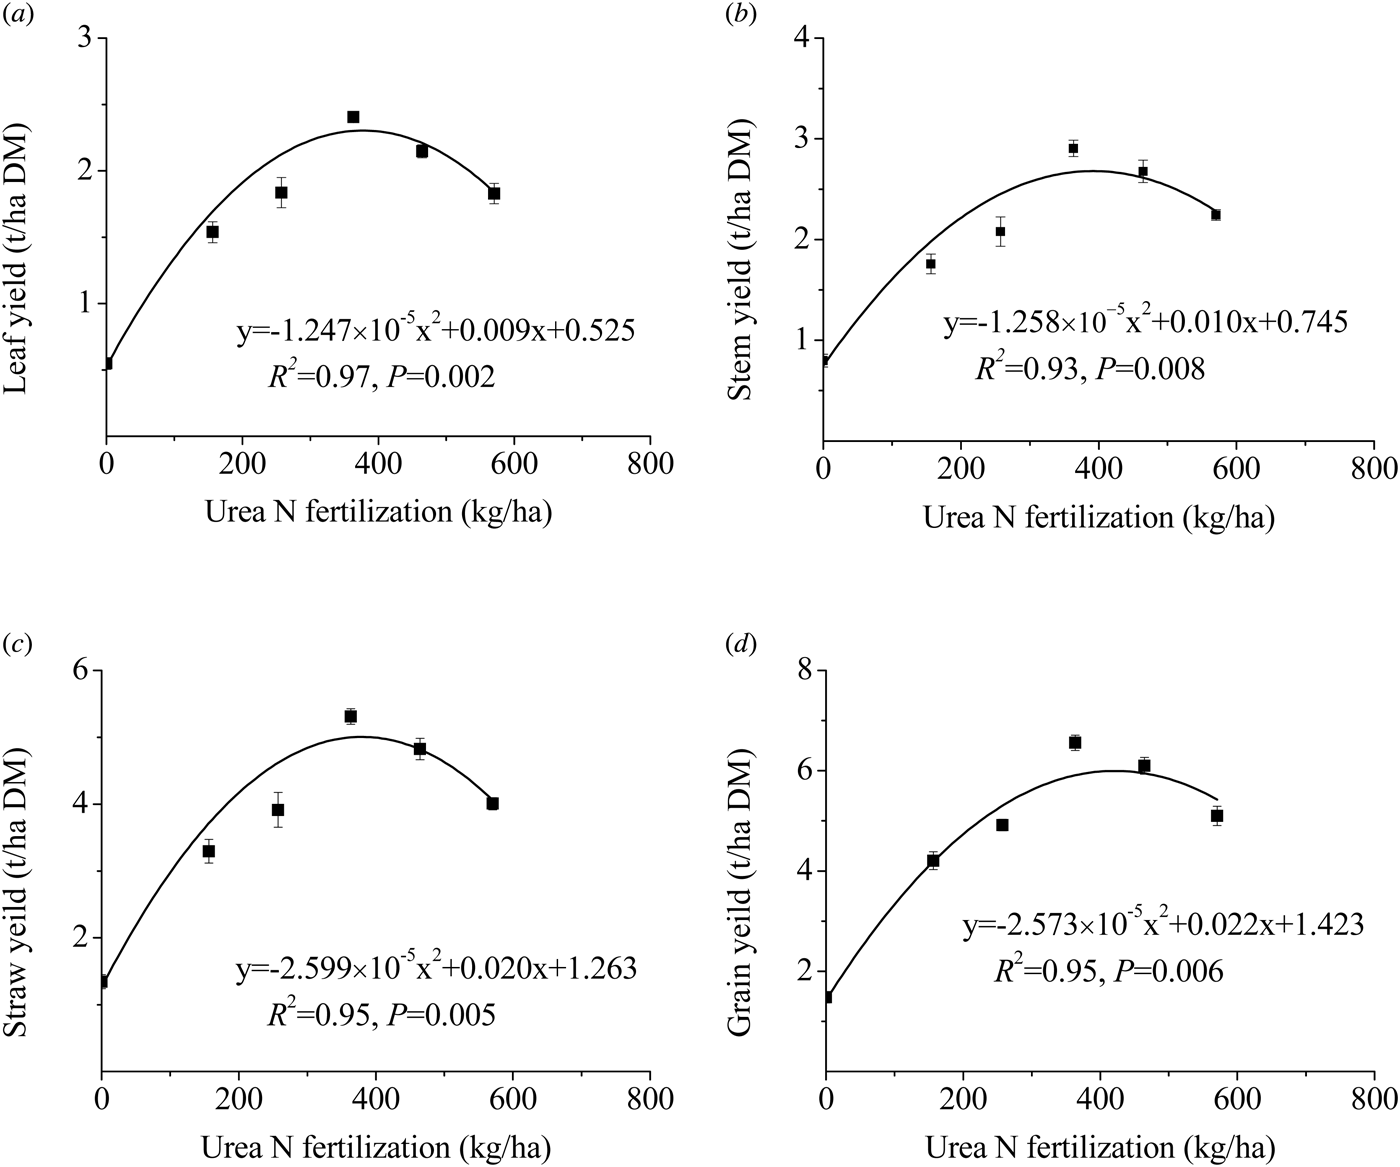
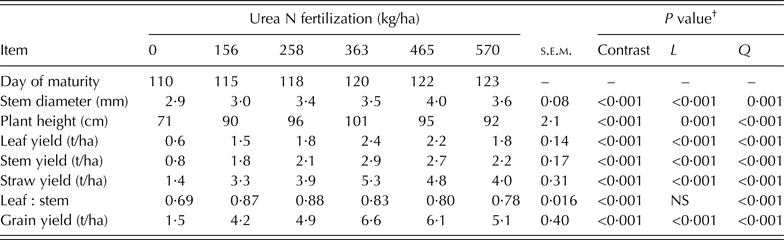
As shown in Table 1, maturity period lasted from 115 to 123 days in response to urea N fertilization. Plant heights were 27–42% higher in the urea N treatments than the control (P < 0·001), and the highest occurred at the urea N level of 363 kg/ha. The urea N fertilization promoted the biomass yields of leaf (150–300% increase), stem (125–263% increase), straw (136–279% increase) and grain (180–340% increase) quadratically (P < 0·001). The biomass yields of leaf (R 2 = 0·97, P = 0·002), stem (R 2 = 0·93, P = 0·008), straw (R 2 = 0·95, P = 0·005) and grain (R 2 = 0·95, P = 0·006) were all increased quadratically with increasing urea N fertilization levels (Fig. 2). A similar response was also observed for leaf : stem ratio (P < 0·001).
Influence of urea N fertilization level on biomass DM yield of leaf (a), stem (b), straw (c) and grains (d) of highland barley harvested at mature stage. Data are mean values with standard error (vertical bars, n = 6).
Influence of urea N fertilization level on growth and biomass yield of highland barley (H. vulgare L. Zangqing 32) on a DM basis*
NS, not significant.
* Highland barley was planted in 36 randomized land blocks (3 × 5 m) per urea N fertilization level, and the number of observations used in the statistical analysis for each urea N level was n = 6.
† Contrast means contrast effect between the zero control and urea N fertilization; L and Q represent linear and quadratic effect of urea N addition, respectively.
Effect of urea nitrogen fertilization level on nutrient accumulation and metabolizable energy of highland barley straw
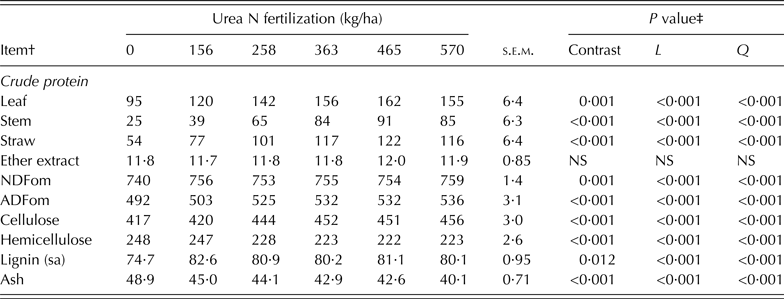
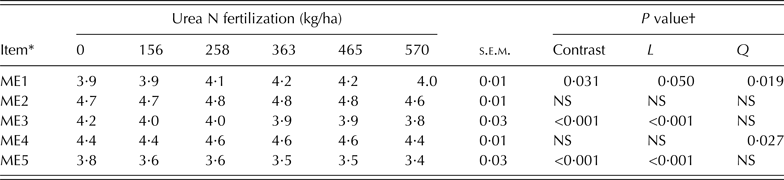
As shown in Table 2, the increase of urea N fertilization increased CP content of leaf, stem and straw quadratically (P < 0·001) and a similar response also occurred for NDF, ADF, cellulose and lignin. The CP accumulation peaked at the urea N level of 465 kg/ha, but NDF, ADF and cellulose accumulation peaked at the urea N level of 570 kg/ha. Conversely, the urea N fertilization decreased ash and hemicellulose contents quadratically (P < 0·001). As shown in Table 3, ME3 and ME5 estimates declined linearly with increasing urea N fertilization (P < 0·05), while ME1 estimates increased quadratically with increasing urea N fertilization (P < 0·001). No significant differences for ME2 and ME4 estimates were observed when urea N fertilization was applied.
Influence of urea N fertilization level on the chemical composition (g/kg DM) of HBS*
NS, not significant.
* Highland barley was planted in 36 randomized land blocks (3 × 5 m) per urea fertilization level, and the number of observations used in the statistical analysis for each urea N level was n = 6.
† NDFom, neutral detergent fibre corrected for residual ash; ADFom, acid detergent fibre corrected for residual ash; Lignin (sa), acid detergent lignin determined by solubilization of cellulose with sulphuric acid.
‡ Contrast means contrast effect between the zero control and urea N fertilization; L and Q represent linear and quadratic effect of urea N addition, respectively.
Influence of urea N fertilization level on metabolizable energy (ME, MJ/kg DM) of HBS
NS, not significant.
* Metabolizable energy (ME) was calculated by applying the following equations (Close & Menke Reference Close and Menke1980; Menke & Steingass Reference Menke and Steingass1988): ME1 = 1·06 + 0·1570 × GP24 + 0·0084 × CP + 0·022 × EE − 0·0081 × ash; ME2 = 2·2 + 0·1357 × GP24 + 0·0057 × CP + 0·0002859 × EE; ME3 = 1·54 + 0·145 × GP24 + 0·00412 × CP + 0·00650 × (CP)2/1000 + 0·0206 × EE; ME4 = 1·56 + 0·1390 × GP24 + 0·007400 × CP + 0·01780 × EE; ME5 = 1·20 + 0·1456 × GP24 + 0·00076575 × CP + 0·01642 × EE in which GP24 is 24 h gas production per 200 mg HBS in DM basis, CP and EE are crude protein and ether extract expressed in g/kg in DM basis.
† Contrast means contrast effect between the zero control and urea N fertilization; L and Q represent linear and quadratic effect of urea N addition, respectively.
Effect of urea nitrogen fertilization on kinetic gas production and end-gas composition
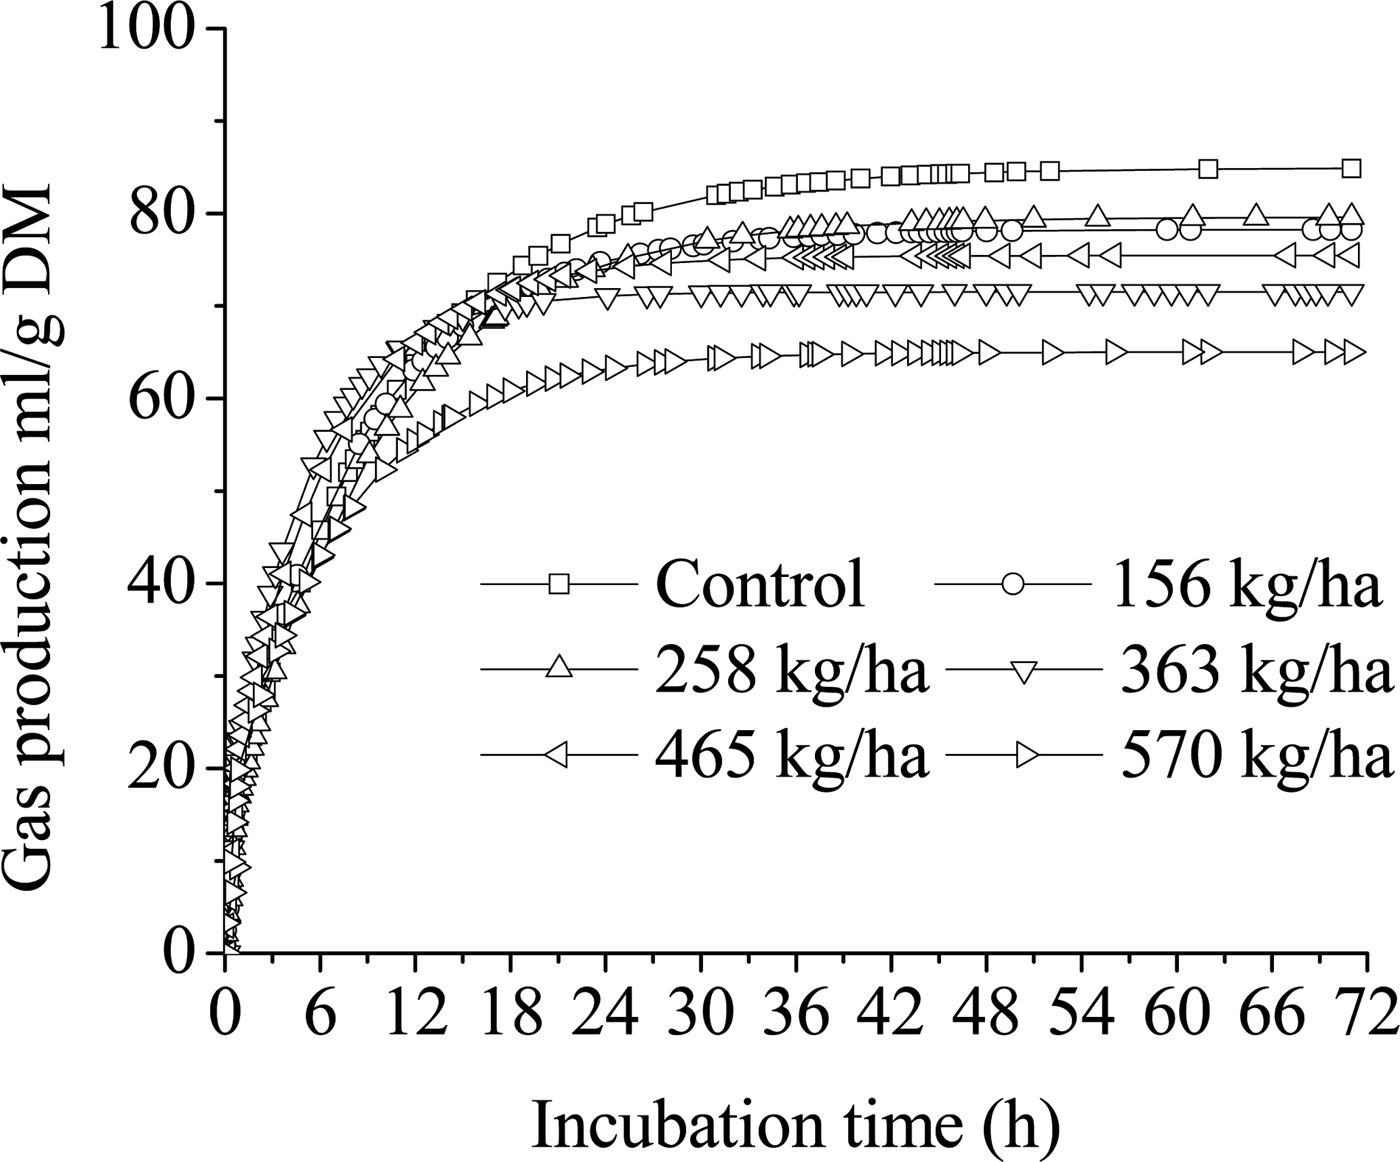
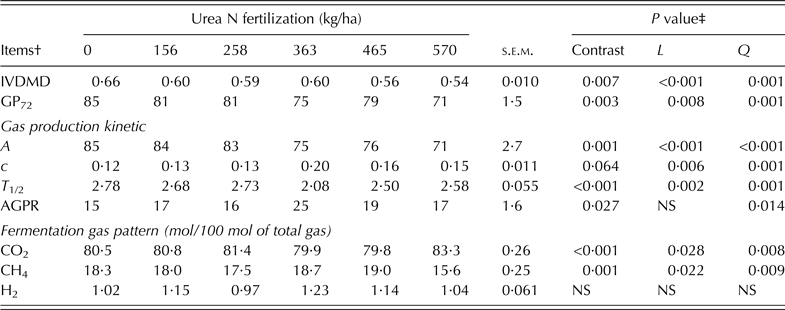
Increasing urea N fertilization decreased in vitro dry matter digestibility (IVDMD) quadratically (P = 0·001). As shown in Fig. 3, cumulative gas production profiles of HBS were influenced by different urea N fertilization rates. In Table 4, both GP72 and A reductions obviously occurred at the urea N fertilization level of ⩾363 kg/ha. The fractional gas production rate (c) increased quadratically with increasing urea N fertilization (P = 0·001), while urea N fertilization linearly decreased T 1/2 (P < 0·001) and quadratically increased AGPR (P = 0·014). Regarding the fermentation end-product gases, urea N fertilization increased molar CO2 proportion (P < 0·001) and decreased molar CH4 proportion (P = 0·001) in comparison with the control, but molar H2 proportion was not affected by urea N fertilization.
Influence of urea N fertilization level on kinetic gas production profiles of HBS incubated with rumen fluid from lactating cows.
Influence of urea N fertilization level on in vitro dry matter digestibilities (IVDMD), kinetic gas production and gas end-products of HBS incubated with rumen fluid from lactating cows*
NS, not significant.
* Diluted buffered rumen fluids (75 ml) were incubated for 72 h with 500 mg ground diet, and the number of observations used in the statistical analysis for each urea N fertilization level per diet was n = 6.
† GP72, cumulative gas production at 72 h; A, the asymptotic gas production; c, the fractional rate for the gas production of ‘A’; T 1/2, the time when half of ‘A’ occurred; AGPR, the average gas production rate when half of ‘A’ occurred.
‡ Contrast means contrast effect between the zero control and urea N fertilization; L and Q represent linear and quadratic effect of urea N addition, respectively.
Effect of urea nitrogen fertilization on fermentation characteristics of highland barley straw
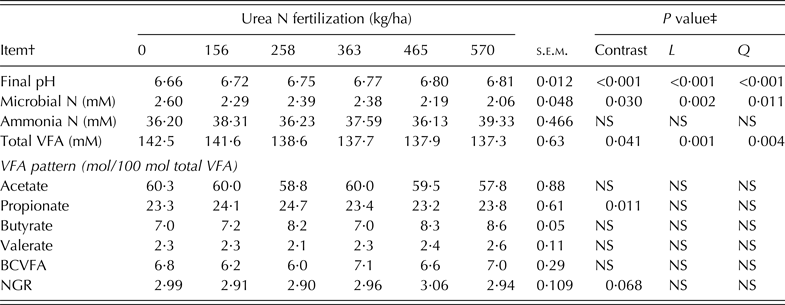
As shown in Table 5, final pH in the culture fluids increased quadratically with urea N fertilization (P < 0·001). The microbial N concentration in the culture fluid decreased with increasing urea N fertilization, but ammonia N concentration was not affected by urea N fertilization in comparison with the control. The urea N fertilization decreased the total VFA concentration quadratically (P = 0·004). Although the urea N fertilization levels tested in the present study did not alter the molar proportions of acetate, butyrate, valerate or BCVFA, molar propionate proportion was markedly increased (P = 0·011). Consequently, NGR tended to decline against the increase of urea N fertilization, although this was not significant (P = 0·068).
Influence of urea N fertilization level on fermentation characteristics in culture fluids of HBS incubated with rumen fluid from lactating cows*
NS, not significant.
* Diluted buffered rumen fluids (75 ml) were incubated for 72 h with 500 mg ground substrate, and the number of observations used in the statistical analysis for each urea N fertilization level per diet was n = 6.
† VFA, volatile fatty acids; NGR, ratio of non-glucogenic to glucogenic acids. BCVFA, Iso-butyrate and iso-valerate were summed as branched-chain volatile fatty acids.
‡ Contrast means contrast effect between the zero control and urea N fertilization; L and Q represent linear and quadratic effect of urea N addition, respectively.
DISCUSSION
Influence of urea nitrogen fertilization on highland barley growth
Nitrogen has been widely accepted as the nutrient most commonly limiting crop production worldwide and is the fertilizer nutrient applied in the greatest amounts (Malhi et al. Reference Malhi, Grant, Johnston and Gill2001). Previous studies have reported urea N fertilizer effects on stem diameter, leaf area index and biomass yield of barley components, in which the prominent feature was the increase of biomass yield with increasing urea N supply (Baethgen et al. Reference Baethgen, Christianson and Lamothe1995; Hansen et al. Reference Hansen, Jørgensen and Thomsen2002; Cantero-Martínez et al. Reference Cantero-Martínez, Angas and Lampurlanés2003; McKenzie et al. Reference McKenzie, Middleton and Bremer2005). Tigre et al. (Reference Tigre, Worku and Haile2014) found that the mature stage of barley growth lasted 3–8 days longer with increasing urea N fertilization rates from 30 to 120 kg/ha. Similarly, maturity was observed to last 5–11 days longer of for highland barley in the present study, suggesting that urea N fertilization promoted vegetative growth and delayed maturity. Fertilizer trials with barley planted at nine locations in Canada showed that straw and grain yield reached 2·5–3·8 and 2·5–3·4 t/ha, respectively, v. ammonium nitrate fertilization rates of 45 and 135 kg N/ha (Bishop & MacEachern Reference Bishop and MacEachern1971). Abeledo et al. (Reference Abeledo, Calderini and Slafer2003) noted that the total grain yield of four barley cultivars grown in Argentina reached 5·2–7 t/ha when urea fertilizer was applied at 350 kg N/ha. McKenzie et al. (Reference McKenzie, Middleton and Bremer2005) tested five urea fertilization rates for nine barley cultivars in southern Alberta, Canada and found that the grain yields of these cultivars were most responsive to urea N fertilization rates from 40 and 160 kg/ha. In agricultural production it is important to give specific advice about fertilization rate depending on different application sites and crop types. It is also necessary for different fertilizers to be given some practical yield response curves, which can be used to improve biomass yield prediction in response to different fertilization rates. Until now, such reference curves for urea N fertilizer are not available for highland barley planted in Tibet. The curves for biomass yield response to urea N application in the present study are shown in Fig. 2, and the HBS and grain maxima yield of 5·0 and 6·0 t/ha were theoretically calculated at optimum urea N levels of 385 and 428 kg/ha, respectively. These levels might be reasonable because the field soil was sandy loam, and the growth period was very rainy in the present study. These urea N rates are higher than the levels reported in the aforementioned studies, suggesting that poor soil fertility at the current experimental site is a key constraint to improving highland barley productivity.
Crops with high soil nutrient supply will show small yield responses to N fertilization and vice versa (Chuan et al. Reference Chuan, He, Pampolino, Johnston, Jin, Xu, Zhao, Qiu and Zhou2013), which could explain why large increments were observed in the present study for plant height (27–42% increase) and biomass yields of leaf (150–300% increase), stem (125–263% increase), straw (136–279% increase) and grain (180–340% increase) of highland barley grown on sandy loam soil with low contents of total nitrogen and total phosphorus. Besides N fertilization level, soil fertility, soil moisture, soil type, the stage of plant growth and climate will also affect plant growth response to N fertilization. Campbell & Davidson (Reference Campbell and Davidson1979) noted that the most important factor influencing grain yield of spring wheat was N fertilizer followed by ambient temperature, while soil moisture stress was the least important, and the results obtained in the present study suggested that a suitable high-N fertilization strategy should be applied to obtain high yield of highland barley in Tibet.
Influence of urea nitrogen fertilization on nutrient accumulation of highland barley straw
Nutrient accumulation response to N fertilization has been reported for common barley in previous studies. For instance, Bishop & MacEachern (Reference Bishop and MacEachern1971) noted that the barley CP content increased by 28% in leaves (from 192 to 245 g/kg CP), by 29% in grain (from 98 to 128 g/kg CP) and by 73% in straw (from 29 to 44 g/kg CP) when the fertilizing rate of ammonium nitrate was increased from 45 and 135 kg N/ha. Increased CP content with increasing N fertilizer amount has also been observed in bluegrass (Poa pratensis L.), tall fescue forage (Festuca arundinacea Schreb.), maize, sweet sorghum and timothy grass (Phleum pratense L.) (Taylor & Templeton Reference Taylor and Templeton1976; Gerrish et al. Reference Gerrish, Peterson, Roberts and Brown1994; da Silva et al. Reference Da Silva, Strieder, da Silva Coser, Rambo, Sangoi, Argenta, Forsthofer and da Silva2005; Almodares et al. Reference Almodares, Jafarinia and Hadi2009; Nordheim-Viken & Volden Reference Nordheim-Viken and Volden2009). Although a similar CP increase was also observed in the present study in response to increasing urea N fertilization rate, the CP content of HBS in Tibet was still quite low compared with those reported in the aforementioned studies at equal N fertilization level. Khorasani et al. (Reference Khorasani, Jedel, Helm and Kennelly1997) noted that the leaf usually had a higher CP content and lower cell wall content than the stem. In contrast, in the present study higher CP contents were observed in leaves and low CP contents in stem. Although the leaf : stem ratio was decreased quadratically by the increase of N fertilization, interestingly, the CP increment observed in the present study was much more in the stem (56–240% increase) than in leaves (26–63% increase), and this could explain why 42–115% CP content was consequently increased in HBS. The results obtained in the present study suggested that urea N fertilization (⩾258 kg/ha) was not only helpful for protein accumulation in HBS but also promoted stem growth of highland barley.
Carbohydrates can be divided into fibre carbohydrates and non-fibre carbohydrates. Fibre carbohydrates consist of cellulose, hemicellulose and a portion of pectin: NDF is a measurement of cellulose, hemicellulose and lignin, and ADF is a measurement of the cellulose and lignin fractions of the plant cell wall while non-fibre carbohydrates consist of sugars, starches and short chains of cellulose-like substrates (Van Soest et al. Reference Van Soest, Robertson and Lewis1991). High accumulation of NDF, ADF and cellulose in response to N fertilization in the present study was also reported for wheat in southern Italy, with a typical Mediterranean environment (De Giorgio et al. Reference De Giorgio, Lestingi, Bovera and Convertini2008). Conversely, Nori et al. (Reference Nori, Abdul Halim and Ramlan2008) reported that urea N fertilization levels from 120 to 240 kg/ha resulted in a linear or quadratic decline in ADF and NDF accumulation in whole rice straw, leaf and stem fractions. Malhi et al. (Reference Malhi, Foster and Gill2003) noted that the ADF content of quack grass (Elytrigia repens L.) was not affected for one cutting, but it showed a slight decrease for two cuttings following ammonium nitrate fertilization ranging from 0 to 168 kg N/ha. Collins et al. (Reference Collins, Brinkman and Salman1990) planted nine adapted oat cultivars with heading dates ranging from early to late in four distinct soil environments of the USA and observed that increasing urea N application rate (0–112 kg/ha) increased plant NDF content (46 g/kg increase) in only one environment, and decreased it slightly in the other three soil environments. The results obtained in the above studies imply that the NDF and ADF accumulation response might vary depending on plant variety, plantation site, fertilizer N source and fertilization level.
An investigation by Gallagher et al. (Reference Gallagher, Hockaday, Masiello, Snapp, McSwiney and Baldock2011) into the fertilization effects of ammonium nitrate at seven rates from 0 to 202 kg N/ha on the quality of maize planted in south-west Michigan, USA, showed that N fertilization increased the lignin content in the grain (86% increase), straw (33% increase) and total plant (49% increase) (Gallagher et al. Reference Gallagher, Hockaday, Masiello, Snapp, McSwiney and Baldock2011). Waramit et al. (Reference Waramit, Moore and Heggenstaller2011) studied the ability of four warm-season grasses including big bluestem (Andropogon gerardii Vitman), eastern gama grass (Tripsacum dactyloides L.), Indian grass (Sorghastrum nutans L. Nash) and switchgrass (Panicum virgatum L.) to enhance cellulose and lignin contents in response to N fertilization rate during 2006 and 2007 near Ames (Iowa, USA). Lemus et al. (Reference Lemus, Brummer, Burras, Moore, Barker and Molstad2008) had previously noted that cellulose and lignin contents of switchgrass planted in southern Iowa, USA, increased linearly, but hemicellulose and ash contents declined linearly with increasing urea and ammonium nitrate fertilization rate. Similarly, the urea N fertilization in the present study also increased the contents of cellulose (by 0·7–9%) and lignin (by 7–10%) and decreased the contents of hemicellulose and ash (by 8–18%). The decreased ash concentration of HBS at increased N fertilization rate could be the result of a simple dilution effect, since the increase in the amount of mineral nutrient taken up by the plant was less than the increase in DM of HBS.
Influence of urea nitrogen fertilization on the digestibility and metabolizable energy of highland barley straw
The plant cell wall fraction in forages has a negative correlation with ruminal digestibility (Jung & Allen Reference Jung and Allen1995) and the decreased IVDMD in response to the increase of urea N fertilization could be caused by cellulose and lignin accumulation of HBS. Similarly, Nori et al. (Reference Nori, Abdul Halim and Ramlan2008) noted that increasing N fertilization level markedly decreased in vitro true organic matter digestibility of the rice stem fraction. Previous studies have also reported that urea N fertilization decreased IVDMD, though it increased CP and NDF contents of tall fescue (Bélanger et al. Reference Bélanger, Gastal and Lemaire1992), vetch grass and legume species (e.g. oat and barley) in the Peruvian highlands (Bartl et al. Reference Bartl, Gamarra, Gómez, Wettstein, Kreuzer and Hess2009). The concomitant increase of fibre and lignin content may play an important role in increasing physical rigidity within secondary cell walls of plant structural tissues. Presumably, the increase in protein accumulation for HBS in the present study could be associated with the proteins linked with fibre in the cell wall, which might not be effectively degraded by rumen microbes in the present study. This assumption can be confirmed by the negative correlation of IVDMD with CP content (R 2 = –0·84, P = 0·033). Almodares et al. (Reference Almodares, Jafarinia and Hadi2009) noted that increasing N fertilization decreased soluble carbohydrate content, though CP content was increased in maize and sweet sorghum fodders.
In vivo ME determination is very expensive and time consuming for individual feedstuffs. According to the relationship between in vivo energy measurement and in vitro fermentability, ME content estimated by the in vitro gas technique has been well established for ruminant animals (Menke et al. Reference Menke, Raab, Salewski, Steingass, Fritz and Schneider1979; Menke & Steingass Reference Menke and Steingass1988). The ME values of HBS in the present study were lower the mean of 7·2–8·4 MJ/kg DM reported for wheat straw (Seker Reference Seker2002) and the mean of 12·99 MJ/kg DM reported for barley straw (Abaş et al. Reference Abaş, Özpinar, Kutay, Kahraman and Eseceli2005) and 11·6–13·1 MJ/kg DM reported for maize stover. The ME values for HBS and their comparisons with the above studies might not be realistic against in vivo determination, and the purpose of these values given in the present study is mainly for comparing different treatments and not for diet formulation. Although urea fertilization increased CP content and decreased ash content, the rise of cellulose and lignin accumulation decreased metabolic gas production, and this could explain the decrease of ME in HBS. The urea N fertilization level of ⩽0·258 kg/ha can be recommended for planting highland barley in Tibet without compromising ME in HBS.
Influence of nitrogen fertilization on fermentation characteristics of highland barley straw
In the present study, the decrease of T 1/2 and the increase of AGPR suggested that urea N fertilization slowed down microbial fermentation, after the soluble fraction of HBS had been quickly digested at an earlier fermentation stage. Previous studies have noted that nitrate content in grass increased due to increasing N fertilizer (Bartholomew & Chestnutt Reference Bartholomew and Chestnutt1977; Mathison et al. Reference Mathison, Okine, McAllister, Dong, Galbraith and Dmytruk1998). The increase of nitrate content has been demonstrated to reduce CH4 emissions in vivo and in vitro (Takahashi & Young Reference Takahashi and Young1991; Sar et al. Reference Sar, Santoso, Zhou, Gamo, Koyama, Kobayashi, Shiozaki, Takahashi, Takahashi and Young2002) and this could explain why CH4 production declined in the present study, though unfortunately nitrate response to increasing urea N fertilization was not determined in the present study. Valk et al. (Reference Valk, Kappers and Tamminga1996) noted that N fertilizer input can reduce water-soluble carbohydrate content. Water-soluble carbohydrates favour glucogenic ruminal fermentation, which consequently reduces CH4 and CO2 emissions (Johnson & Johnson Reference Johnson and Johnson1995).
The final pH value in cultural fluids was increased by N fertilization in the present study, but remained within the normal rumen pH range of 6·4–6·8 (Jouany Reference Jouany2006). Chanthakhoun et al. (Reference Chanthakhoun, Wanapat and Berg2012) noted that a higher level of CP (124–181 g/kg CP) improved ammonia N and microbial CP synthesis in swamp buffalo. Conversely, though the CP content of HBS in the present study was increased by urea N fertilization, the fermentation of HBS presented a decrease of microbial N and no change in ammonia N was observed. This was possibly because rumen microbes might not effectively digest and metabolize the CP content of HBS. Besides ammonia N, amino acids taken up by the micro-organisms can be incorporated into microbial protein when supplies of fermentable carbohydrates are readily available in the rumen (Miller et al. Reference Miller, Moorby, Davies, Humphreys, Scollan, MacRae and Theodorou2001). Previous studies have reported that N fertilization markedly decreased the water-soluble carbohydrate content (e.g. sugars, starch and fructan) by ⩽50% (Blaser Reference Blaser1964; Jones et al. Reference Jones, Ap Griffith and Walters1965; Wilman & Wright Reference Wilman and Wright1978; Keating & O'Kiely Reference Keating and O'Kiely2000; Adesodun et al. Reference Adesodun, Mbagwu and Oti2001). If the water-soluble carbohydrate availability is relatively low, both the balance and the temporal utilization of N and energy-yielding components could be out of phase. Consequently, reduced microbial N utilization will, in turn, lead to a reduction in microbial digestion and fermentation.
Previous studies noted that rapid starch fermentation in the rumen led to increased production of VFA and a reduction in ruminal pH (Nagaraja & Titgemeyer Reference Nagaraja and Titgemeyer2007; Davies et al. Reference Davies, McKinnon and Mutsvangwa2013). Non-starch polysaccharides and fibre are also fermentable to produce VFA as energy source for ruminant animals. In the present study, the decrease of total VFA implied that the microbial fermentability of HBS was decreased with increasing N fertilization, and this could explain the decreased IVDMD in response to higher accumulation of cellulose and lignin. The lack of response for acetate, butyrate, valerate and BCVFA in molar proportions implies that the fermentation pathways including the lactic acid and acetone–butanol fermentation pathways were not changed, and rumen micro-organism composition might not be affected since different microbes generate different VFA end-products. Propionate formation occurs mainly via succinate and an alternative pathway involving acrylate, such as succinate and acrylate pathway, is also operative. It has been widely accepted that starch-rich diets favour the development of propionate-producing bacterial species which are associated with an increase in the proportion of molar propionate (France & Dijkstra Reference France, Dijkstra, Dijkstra, Forbes and France2005). Previous studies have also noted that cellulose fermentation favours high propionate production in batch cultures (John et al. Reference John, Barnett and Reid1957; Beuvink & Spoelstra Reference Beuvink and Spoelstra1992), so the cellulose accumulation of HBS could explain why the urea N fertilization increased molar propionate proportion in the present study.
In summary, increasing the level of urea N fertilization resulted in late maturation of highland barley and increased both grain and straw yield. Although urea N fertilization markedly increased protein accumulation in HBS, the increase of cellulose and lignin contents presented a much more detrimental impact on the digestibility and fermentability of HBS. A urea N fertilization rate of ⩽385 kg/ha can be recommended for planting highland barley in Tibet without reducing energy and digestibility of HBS.
The present study was funded by the Research and Demonstration on Key Techniques of Safety Growing and Efficient Use of Forage Grass in One River, Two Streams Areas in Tibet of China (Project no. Z2013C02N02), the Importation and Development of High-Caliber Talents Project of Beijing Municipal Institutions (Project no. CIT&TCD20130324) and Tibet Natural Science Fund (Project no. 2013ZR13-67). The authors also appreciate Y. H. Zhang, Y. X. Fang and R. H. Guo for their assistance in sample collection and chemical analysis, etc.