


Introduction
The potential of arthropod predators to suppress pest populations has been thoroughly established by recent literature reviews (Chang & Kareiva, Reference Chang, Kareiva, Hawkins and Cornell1999; Gurr & Wratten, Reference Gurr and Wratten2000; Symondson et al., Reference Symondson, Sunderland and Greenstone2002). However, the challenges for studying predator–prey interactions under field conditions are formidable (Greenstone & Morgan, Reference Greenstone and Morgan1989; Sunderland, Reference Sunderland1999); and, in any given system, it can be difficult to determine the contribution of specific predator species to pest population suppression.
Predation data may be obtained by direct observation, by gut analysis or by experimental field manipulations (Sunderland, Reference Sunderland1988; Greenstone, Reference Greenstone1999). Of these, the least disruptive to ecosystem processes is gut analysis, because it requires only short, intermittent presences in the field by the investigator to collect the predators, after which gut analysis proceeds in the laboratory. For predators with chewing mouthparts, chiefly earwigs (Dermaptera) and adult carabid and staphylinid beetles, it is possible – though tedious! (Sunderland, Reference Sunderland1975; Triltsch, Reference Triltsch1999) – to identify prey remains by microscopic analysis of hard parts in the dissected gut (Sunderland et al., Reference Sunderland, Crook, Stacey and Fuller1987; Holopainen & Helenius, Reference Holopainen and Helenius1992; Triltsch, Reference Triltsch1999). However, most terrestrial arthropod predators are fluid feeders, and for the majority of predator–prey systems a molecular approach to gut analysis will be necessary to assess all interactions.
Two technological approaches have dominated molecular gut-content analysis: serological methods, with monoclonal antibody-based assays to detect prey antigenic determinants representing the state of the art (Greenstone, Reference Greenstone, Symondson and Liddell1996; Symondson et al., Reference Symondson, Erickson and Liddell1999; Harwood et al., Reference Harwood, Sunderland and Symondson2004); and polymerase chain reaction (PCR; Ehrlich, Reference Ehrlich1989) amplification of prey deoxyribonucleic acid (DNA) sequences (Symondson, Reference Symondson2002; Sheppard & Harwood, Reference Sheppard and Harwood2005). Where prey stage-specificity is not required, PCR-based assays are preferred, due to the ease of designing primers and disseminating the technology to other practitioners, who can have their own primer sets developed for a fraction of the time and cost of a monoclonal antibody (Zaidi et al., Reference Zaidi, Jaal, Hawkes, Hemingway and Symondson1999; Chen et al., Reference Chen, Giles, Payton and Greenstone2000; Hoogendoorn & Heimpel, Reference Hoogendoorn and Heimpel2001).
Given the versatility of predatory behaviour and the subtle complexities of trophic relationships (Sunderland, Reference Sunderland1999; Juen & Traugott, Reference Juen and Traugott2005), data derived from gut analysis must be analysed with great care. For example, remains detected in the gut of a particular predator may not reflect predation by that predator on a live prey item, but rather scavenging on an already-dead animal (Calder et al., Reference Calder, Harwood and Symondson2005; Foltan et al., Reference Foltan, Sheppard, Konvicka and Symondson2005) Alternatively, it might represent predation on another predator that had killed and consumed that prey animal (so-called ‘secondary predation;’ Harwood et al., Reference Harwood, Phillips, Sunderland and Symondson2001; Sheppard et al., Reference Foltan, Sheppard, Konvicka and Symondson2005).
The detectability half-life
The time during which prey remains are detectable in the gut of a predator, whether by serological or by PCR assay, is an important consideration in the interpretation of molecular gut-content analysis data. Obviously, detectability of prey material within the predator will diminish as it is digested. If the decay rate of detectability is exponential, then the detectability half-life, defined as the time after which only half of the meals consumed can be detected, is an appropriate standardized measure of the detectability interval (Greenstone & Hunt, Reference Greenstone and Hunt1993). The exponential model has generally fit molecular gut-content analysis data cast in this form very well, whether the targets of the assay are protein or DNA molecules of the prey (Fichter & Stephen, Reference Fichter and Stephen1981; Greenstone & Hunt, Reference Greenstone and Hunt1993; Hagler & Naranjo, Reference Hagler and Naranjo1997; Chen et al., Reference Chen, Giles, Payton and Greenstone2000; Wallace, Reference Wallace2004; Ma et al., Reference Ma, Li, Keller, Schmidt and Feng2005; Fournier et al., Reference Fournier,, Hagler, Daane, de Leon, Groves, Costa and Henneberry2006; Read et al., Reference Read, Sheppard, Bruford, Glen and Symondson2006; Juen & Traugott, Reference Juen and Traugottin press).
The rate of decay in detectability, and hence the half-life, is likely dependent on many variables, including ambient temperature and age and size of the prey and predator (Hagler & Naranjo, Reference Hagler and Naranjo1997; Hoogendoorn & Heimpel, Reference Hoogendoorn and Heimpel2001), and feeding mode and digestive physiology of the predator. Here we examine the influence on half-life of differences in feeding mode and digestive physiology, by determining it for a single prey species in two predators that differ dramatically in these attributes.
The Colorado potato beetle and its predators
The Colorado potato beetle, Leptinotarsa decemlineata (Say) (Coleoptera: Chrysomelidae), is one of the most important pests of potato and other solanaceous crops in the temperate regions of the Northern Hemisphere. First recorded on potato in Nebraska in the mid 19th century, it quickly spread to the eastern USA and Canada and appeared in France in 1922. It is now found in continental Europe, Turkey, Iran, central Asia and western China (Weber, Reference Weber2003). It has tremendous biotic potential and physiological versatility, facilitating the rapid evolution of resistance to most classes of insecticides, including the widely used neonicotinoid pesticides imidacloprid and thiamexotham, and the novel compound spinosad (Zhao et al., Reference Zhao, Grafius and Bishop2000; Byrne et al., Reference Byrne, Grafius, Bishop and Pett2004; Mota-Sanchez et al., Reference Mota-Sanchez, Hollingworth, Grafius and Moyer2006).
A number of generalist predators have been observed feeding on L. decemlineata in the field in North America (Ferro, Reference Ferro, Zehnder, Powelson, Jansson and Raman1994). The coccinellid Coleomegilla maculata (DeGeer) (Coleoptera: Coccinellidae) is often the most abundant generalist predator on foliage in potato fields (Benton & Crump, Reference Benton and Crump1981; Hazzard et al., Reference Hazzard, Ferro, van Driesche and Tuttle1991; Hilbeck et al., Reference Hilbeck, Eckel and Kennedy1997) and may kill more than half the L. decemlineata eggs in a generation (Groden et al., Reference Groden, Drummond, Casagrande and Haynes1990; Hazzard et al., Reference Hazzard, Ferro, van Driesche and Tuttle1991), as well as many of the small larvae. Although less abundant, the pentatomid Podisus maculiventris (Say) (Hemiptera: Pentatomidae) is commonly part of the generalist predator complex in potato fields (Hazzard et al., Reference Hazzard, Ferro, van Driesche and Tuttle1991; Heimpel & Hough-Goldstein, Reference Heimpel and Hough-Goldstein1992; Ferro, Reference Ferro, Zehnder, Powelson, Jansson and Raman1994), consumes eggs and larvae of L. decemlineata in the field (Hough-Goldstein & McPherson, Reference Hough-Goldstein and McPherson1996; Tipping et al., Reference Tipping, Holko, Abdul-Baki and Aldrich1999) and has great potential to suppress Colorado potato beetle populations when appropriately managed (Hough-Goldstein & McPherson, Reference Hough-Goldstein and McPherson1996; Aldrich & Cantelo, Reference Aldrich and Cantelo1999). Both predators are highly polyphagous and also omnivorous, feeding on pollen (C. maculata) and other plant tissues (Coll & Guershon, Reference Coll and Guershon2002).
Coleomegilla maculata uses its mandibles to macerate its prey, ingesting the resultant solid and fluid fractions into the gut without extra-oral enzymatic digestion (Butt, Reference Butt1951; Jonathan Lundgren, personal communication). In P. maculiventris, the mandibular stylets bear back-curved teeth that enable it to harpoon and hold the prey, and then to insert the stylets deep into all regions of the body to lacerate organs (Cohen, Reference Cohen1990). The animal then employs non-refluxing extra-oral digestion, injecting salivary amylase, hyaluronidase, lipases and proteinases to disrupt the intracellular matrix and basement membranes of prey tissues (Cohen, Reference Cohen1990, Reference Cohen1998) prior to ingestion through the narrow mouthparts into the gut, where intracellular digestion takes place. Because of the contrast in how they handle prey prior to ingestion, we expected these two predators to have markedly different detectability half-lives for remains of the same prey.
Here we derive half-lives for L. decemlineata DNA in the guts of C. maculata and P. maculiventris under simulated field conditions. Using field data, we then show why such estimates are essential to provide an accurate assessment of their importance as agents of biological control.
Materials and methods
Prey insects
Leptinotarsa decemlineata came from a colony at the USDA-ARS Insect Biocontrol Laboratory that originated from eggs provided by the New Jersey Department of Agriculture in 1996 with field-collected insects from potato fields at the USDA-ARS Beltsville Agricultural Research Center (BARC) in Beltsville, Maryland, introduced yearly to maintain genetic diversity. Adults and larvae were fed potato foliage (cv. Kenebec), and maintained in the laboratory under a photoperiod regime of 16:8 (L:D) with approximately 50% relative humidity (RH) at approximately 25°C. Moistened ProMix (Premier Horticulture, Inc., Quakertown, Pennsylvania, USA) was provided as a medium for pupation.
The false potato beetle, Leptinotarsa juncta (Germar), which ranges through the South Atlantic and West South–Central USA (Riley et al., Reference Riley, Clark and Seeno2003) and can co-occur with L. decemlineata either on potatoes or on horsenettle (Solanum carolinense L.) on the margins of, or within, potato fields, was used as a negative control for the assay. It was also used as a sustaining food item to support normal predator metabolism during L. decemlineata DNA half-life studies. Beetles were collected in 2003 from S. carolinense in grazed pastures at the Burgundy Center for Wildlife Studies in Hampshire County, West Virginia, and in 2004 from the same plant species at BARC. They were maintained in a growth chamber on greenhouse-raised S. carolinense under a 16:8 photoperiod at 25°C and 50±10% RH, and provided with moistened ProMix for pupation. A variety of other Leptinotarsa populations (table 1) were also sampled in order to inform primer design, and 1–5 individuals from each population subjected to PCR with L. decemlineata and L. juncta primers to verify species-specificity of the PCR assay.
Collecting localities and number of individuals sequenced for additional Leptinotarsa populations subjected to PCR with the L. decemlineata and L. juncta primers.

To guard against false positives from members of other genera, we also tested the following species, which were at least occasionally seen in the field and are potential prey items: Epilachna varivestis Mulsant (Coleoptera: Coccinellidae); Diabrotica undecimpunctata howardi Barber, Epitrix cucumeris (Harris), Acalymma vittatum (F.), and Lema trilinea White (Coleoptera: Chrysomelidae); Oebalus pugnax (F.) and Euschistus servus euschistoides (Vollenhoven) (Hemiptera: Pentatomidae); Orius insidiosus (Say) (Hemiptera: Anthocoridae); Geocorus punctipes (Say) (Hemiptera: Lygaeidae); Macrosiphum euphorbiae (Thomas) (Hemiptera: Aphididae); and Empoasca fabae (Harris) (Hemiptera: Cicadellidae).
In order to standardize the quantity of DNA consumed by an individual, a single egg of L. decemlineata was used as the prey item for half-life determination.
Predatory insects
In order to standardize predators for feeding studies, we chose third instars, which are large enough to completely consume one L. decemlineata egg without becoming satiated. They were taken from long-term colonies so that we could obtain cohorts that would be in similar physiological state. To establish colonies, adults were collected in the field at BARC, mated in the laboratory and maintained under the same growth chamber conditions as L. juncta. Both species had been in colony for two years at the time of the experiments.
Coleomegilla maculata were collected by hand from corn and potato fields. As many as eight adults were grouped in 300 ml ice cream cups, with two moistened dental wicks, 0.6 ml of pollen substitute (Bee-PRO, Mann Lake Ltd, Hackensack, Minnesota, USA) and at least one L. decemlineata egg mass. After one week, mating pairs were placed in 200 ml rearing cups with one moistened dental wick, 50 μl pollen substitute and one L. decemlineata egg mass. Neonates were provided with 30–40 μl of Helicoverpa zea Boddie (Lepidoptera: Noctuidae) eggs (Benzon Research, Inc., Carlisle, Pennsylvania, USA) and switched to L. decemlineata egg masses once they reached the third instar.
Adult P. maculiventris were collected in pheromone traps (Aldrich & Cantelo, Reference Aldrich and Cantelo1999) at the edge of a deciduous forest. Six to ten adults were held in plastic cages (20×27×10 cm), provided with mealworms, green beans, saturated water wicks and shredded paper as a substrate for the egg laying. Eggs were removed at least twice per week and placed in 80 mm Petri dishes with green beans and a soaked dental wick. Second stage nymphs were additionally supplemented with mealworms for the rest of the growth cycle.
Individuals of the predators, Harmonia axyridis (Pallas) and Coccinella septempunctata L. (Coleoptera: Coccinellidae) and Perillus bioculatus F. (Hemiptera: Pentatomidae), all of which were common in the plots, were collected in the field and subjected to PCR with the L. decemlineata, C. maculata, and P. maculiventris primers to ensure that they would not produce false positives in the gut-content assays.
Feeding studies to determine L. decemlineata DNA detectability half-life
All predators were starved before the experiment for a period sufficient to stimulate them to feed reliably. This took 48 h for P. maculiventris, but 24 h was sufficient for C. maculata, which in any event could not tolerate more than 24 h starvation without becoming visibly dehydrated. Each third instar larva or nymph was placed individually in a 35 mm Petri dish and provided with one quarter of a cotton dental wick that had been saturated with diH2O. They were placed overnight in an incubator programmed to simulate mean hourly temperatures 15 cm above the soil surface in a BARC potato field during the last two weeks of May 2003 (BARC, 2003), with a photoperiod of 15:9 L:D and 50±5% RH with the lights on at 0600 h and off at 2100 h. Feeding trials were begun on the following day at 1000 h, a time of observed high activity levels in the field for C. maculata (Mack & Smilowitz, Reference Mack and Smilowitz1980; Benton & Crump, Reference Benton and Crump1981); diel periodicity has not been studied in P. maculiventris, but it is generally considered to be diurnal (R. J. O'Neil, personal communication) and is abroad in daylight in potato fields (Hazzard et al., Reference Hazzard, Ferro, van Driesche and Tuttle1991).
Each C. maculata larva or P. maculiventris nymph was fed a single L. decemlineata egg and observed until it had consumed it; those that had not consumed the egg within 2 h were dropped from the experiment. Except at the 16 h time point for P. maculiventris, for which only 13 animals could be induced to feed, 20 individuals of each predator species were harvested at each of six time points: 0, 4, 8, 12, 16 and 20 h (because this was insufficient to determine the half-life for P. maculiventris, we added 48 and 72 h time points for that species). Those in the t=0 h group were frozen at −20°C immediately after consuming the egg. For those designated for later time points, any remaining L. decemlineata egg chorion was removed. At that point each animal received 3–5 L. juncta eggs and was returned to the incubator. Those to be killed at 4 or 8 h post-feeding received three eggs, those in the 12 and 16 h groups received four eggs, and those in the 20, 48, and 72 h groups received five eggs; the maximum number consumed by any individual was four eggs (L. juncta eggs have approximately 1.8× the wet mass of L. decemlineata eggs; Weber et al., Reference Weber, Rowley, Greenstone and Athanas2006). At the designated time point, each remaining predator larva or nymph was removed from the incubator and frozen at −20°C.
DNA procedures
DNA extraction and purification were performed according to the protocols of Greenstone et al. (Reference Greenstone, Rowley, Heimbach, Lundgren, Pfannenstiel and Rehner2005). Preliminary PCRs (30 μl) for nucleotide sequencing of cytochrome oxidase I (COI) were performed in Buffer B (Promega, Madison Wisconsin, USA), with 1 mm dNTPs (Promega), 10 nm primers C1-J-1751 and C1-N-2191 (Simon et al., Reference Simon, Frati, Beckenbach, Crespi, Liu and Flook1994), 40 μg ml−1 RNAse A (Promega), 1% PVP MW 40 000 (Fisher Scientific, Pittsburgh, Pennsylvania, USA), 0.2% BSA (Sigma, St Louis, Missouri, USA), 0.1 unit μl−1 Taq polymerase (Promega) and 4.5 mm MgCl2 (Promega). Initial denaturation was for 3 min at 94.5°C, followed by 40 cycles of 45 sec at 94.5°C, 1 min at 37°C, and 2 min at 72°C; 5 min at 72°C completed the program. Conditions for species-specific amplifications were the same as for preliminary amplifications, except that MgCl2 was at 2.0 mm, extension time was 1.0 min, and annealing temperatures were between 53°C and 55°C, depending on the species to be amplified (table 2).
Primer sequences (5′–3′).
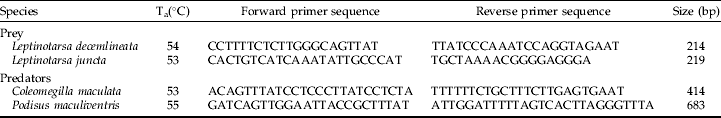
Ta, annealing temperature. Size, size of amplicon.
The success of each reaction was checked by electrophoresis of 6 μl of the PCR/Stop reaction in 1.5% agarose (preliminary reactions) or 2.25% agarose (species-specific reactions) in 0.5× TAE. The remainder of the reaction was loaded and the fragments for sequencing were excised from 1.5% NuSieve agarose (Cambrex Bio Science Rockland Inc., Rockland, Maine, USA) run in 1× TAE modified to have a final EDTA concentration of 0.1 mm. Sequencing was by BigDye terminator v3.1 kits on an ABI 3100 sequencer (Applied Biosystems, Foster City, California, USA). Editing, alignments and primer design were performed with Lasergene (DNAStar, Madison, Wisconsin, USA). Primer sequences, annealing temperatures and amplicon size for the species-specific PCR reactions are given in table 2.
Each PCR reaction included two positive (L. decemlineata) controls, two positive fed predator (t=0) controls, two negative (L. juncta) controls, two starved predator controls, and one no-DNA control. Additionally, control PCR reactions were run on all samples to verify that the DNA in the samples was amplifiable. For the half-life experiments, the control reactions were the predator-specific reactions; control reactions for the field samples employed generic CO I primers (Simon et al., Reference Simon, Frati, Beckenbach, Crespi, Liu and Flook1994).
Statistical analysis
Half-lives for DNA detectability were determined by the PROC PROBIT Procedure (SAS Institute, 1999) and tested for statistical significance by the method of Payton et al. (Reference Payton, Greenstone and Schenker2003).
Collection of predators from the field
Between 1 June and 29 July 2005, during the hours of 0930–1700 h, 36 C. maculata (34 adults and 2 larvae) and 32 P. maculiventris (27 adults and 5 nymphs) were collected by hand from Colorado potato beetle-infested foliage from the central portions of a 0.4 ha potato field at BARC and immediately placed into 80% EtOH for assay with our L. decemlineata primers. The field comprised a mosaic of conventionally-tilled and rye-mulched plots, surrounded by fields of maize, soybeans, alfalfa hay and mixed hardwood forest.
Sequences
COI sequences derived in this research were deposited in GenBank: C. maculata No. AY615732; L. decemlineata No. AY613926; L. juncta Nos. AY531755 (Maryland) and AY531756 (West Virginia); L. haldemani No. DQ4593776; and P. maculiventris No. DQ459378.
Results
The specific PCR primers developed to detect DNA of L. decemlineata and L. juncta produced the expected bands of 214 and 219 bp, respectively (fig. 1). The L. decemlineata primers correctly identified all sampled populations of that species, and the L. juncta primers correctly identified both populations of that species; neither primer set amplified L. lineolata or L. haldemani DNA (L. haldemani data not shown).
Gel showing specificity of PCR primers for Leptinotarsa decemlineata and L. juncta. Lanes 1, 15, and 29, DNA ladder (bright band is 500 bp); lanes 14 and 28, DNA-free control; Lanes 2–14, L. decemlineata primers; lanes 16–28, L. juncta primers. Lanes 2 and 16, L. decemlineata, colony; lanes 3 and 17, L. juncta, West Virginia; lanes 4 and 18, L. decemlineata, Michigan; lanes 5 and 19, L. decemlineata, Nebraska; lanes 6, 20, L. decemlineata, Texas; lanes 7 and 21, L. decemlineata, Kansas; lanes 8 and 22, L. decemlineata, Idaho; lanes 9 and 23, L. decemlineata, Arivaca, Arizona; lanes 10 and 24, L. decemlineata, Patagonia, Arizona; lanes 11 and 25, L. decemlineata, Hurlock, Maryland; lanes 12 and 26, L. juncta, Beltsville, Maryland; lanes 13 and 27, L. lineolata, Patagonia, Arizona.

Half-lives for detecting the DNA of a single L. decemlineata egg were estimated as 7.0 h for C. maculata and 50.9 h for P. maculiventris (fig. 2). These half-lives are statistically different (P<0.05; 95% fiducial limits 6.74 and 25.16, and 35.53 and 90.76, respectively). The slopes for both predator species are significantly different from zero (Chi-square=43.36 and 16.94, respectively, df=1, P<0.0001). Fit of the probit model is excellent for Coleomegilla but relatively weak for P. maculiventris (table 3); it is obvious from inspection of fig. 2 that this is due to the behaviour of the data between 4 and 16 h.
Results of the feeding experiments. Symbols are PCR data; n=20 individual predators assayed for each data point, except for t=16 h of Podisus maculiventris, for which n=13. Lines are fitted probit model with 95% fiducial limits. Filled diamonds and solid lines, Leptinotarsa decemlineata DNA in Coleomegilla maculata fed a single L. decemlineata egg; filled circles and dotted lines, L. decemlineata DNA in Podisus maculiventris fed a single L. decemlineata egg. Open diamonds, L. juncta DNA in the same C. maculata individuals fed L. juncta eggs after time zero; open circles, L. juncta DNA in the same P. maculiventris individuals fed L. juncta eggs after time zero.

Goodness of fit tests of the probit model for probability of detecting DNA from a single Leptinotarsa decemlineata egg vs. hours since feeding.
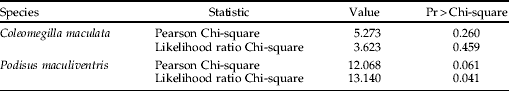
DF=4 in all cases.
We were able to detect L. juncta DNA in 80–100% of the animals that had been offered eggs of that species after time zero (fig. 2), indicating that we can detect L. decemlineata in the presence of interfering DNA from another species that is an alternate prey item for these predators.
Six of the 36 C. maculata and 15 of the 32 P. maculiventris collected from potato foliage in 2005 tested positive for L. decemlineata DNA. Identity of the immatures, which were found in association with other coccinellid and pentatomid species in potato fields at BARC, was verified by PCR using the species-specific primers for predators in table 2.
Discussion
Our PCR assay detects remains of the Colorado potato beetle in the guts of predators that belong to different insect orders and are also significant members of the generalist predator complex in potato fields throughout the USA. Further, we can distinguish them in the gut from those of a Colorado potato beetle congener that is likely to be an alternate prey item for these predators (we see it on both potato and horsenettle foliage in and around potato fields at BARC), as well as from the myriad other potential prey in the potato field, an important consideration in any predator–prey system (Admassu et al., Reference Admassu, Juen and Traugott2006). The weak fit of the exponential model to the half-life data for P. maculiventris (fig. 2) is puzzling, but weak fit in the first few time points of a half-life determination is not unprecedented (Hagler & Naranjo, Reference Hagler and Naranjo1997; de León et al., Reference De León, Fournier, Hagler and Daane2006; Juen & Traugott, Reference Juen and Traugottin press).
The goal of the development of molecular gut-content analysis is to provide tools for assessing the impact of predators on prey populations. Much has been written about the quantitation of gut-content analysis data, for which the Holy Grail is an estimate of the number of prey eaten per unit time. The only investigator to approach this milestone has been J.P. Dempster, who, because the interval between meals was larger than the half-life of the only assay then available (the precipitin test), could defend the assertion that a positive assay for prey remains represented only a single prey item in a predator's gut (Dempster, Reference Dempster1960). In all subsequent investigations, our inability to know simultaneously the contributions of time since feeding, number of prey eaten and size of prey eaten, to the detectability of prey remains has prevented conversion of samples of positives in predator gut-content assays to estimates of number of prey eaten per unit time by a predator population (Sopp et al., Reference Sopp, Sunderland, Fenlon and Wratten1992).
Hoogendoorn & Heimpel (Reference Hoogendoorn and Heimpel2001) made ingenious use of the inverse correlation between amplicon size and detectability half-life to estimate the time since feeding for C. maculata consuming eggs of Ostrinia nubilalis (Hübner) (Lepidoptera: Crambidae). They note, however, that the method would be inaccurate if meals contained varying amounts of DNA. Similarly, the mean number of prey items in the gut represented by a sample of gut-content assay positives can be estimated with a statistical model (Nakamura & Nakamura, Reference Nakamura and Nakamura1977; Greenstone, Reference Greenstone1979; Lister et al., Reference Lister, Usher and Block1987), but this alone would not translate to a rate of feeding without knowledge of the feeding interval and size of the prey item.
Finally, the quantity of prey DNA or protein in the gut can be estimated by ELISA or quantitative PCR. This quantity may decay exponentially with time (Fichter & Stephens, Reference Fichter and Stephen1981; Sopp & Sunderland, Reference Sopp and Sunderland1989; Harwood et al., Reference Harwood, Phillips, Sunderland and Symondson2001; Fournier et al., Reference De León, Fournier, Hagler and Daane2006), enabling estimation of a half-life for prey remains (Symondson & Liddell, Reference Symondson and Liddell1995). It is important to understand that although the decay of prey remains with time is of the same form as the decay of detectability, it does not measure the same thing. Consequently, the half-life for prey remains is not the same as the detectability half-life, and does not have the same application to gut-content data analysis: to provide a predator-species-specific standard of comparison for the value of a positive by removing the bias that would otherwise overvalue the role of predator species with longer detectability periods (Sopp et al., Reference Sopp, Sunderland, Fenlon and Wratten1992; Chen et al., Reference Chen, Giles, Payton and Greenstone2000; Fournier et al., Reference De León, Fournier, Hagler and Daane2006).
This is well illustrated by the analysis of our field-collected predators. The raw data on the incidence of L. decemlineata DNA in these animals suggest that P. maculiventris, with 46.9% positives, has more than three times the impact per predator on the Colorado potato beetle population at BARC than C. maculata, with only 15.4% positives. However, when the difference in half-lives is taken into account, C. maculata's relative impact increases, since the detectability of DNA from a single L. decemlineata egg is always longer in P. maculiventris than in C. maculata (fig. 2). Specifically, the ratio of depicted detectabilities ranges from just over 1 at t=0 h to nearly 90 at t=20 h. Therefore, whereas the raw data would lead one to believe that the per capita impact of C. maculata on the L. decemlineata population is only about one-third that of P. maculiventris, the detectability-weighted data show that the per capita impact of C. maculata would have been underestimated, and could even be greater than that of P. maculiventris, depending upon the distribution of times since feeding in the field. The approach of Hoogendoorn & Heimpel (Reference Hoogendoorn and Heimpel2001), coupled with field observations of the time frequency of predation events, would enable us to delimit the universe of possible times since feeding for each predator.
Although the decay of detectability has been found to be exponential in numerous studies, there are relatively few actual half-life estimates in the literature. In table 4, we provide references that report molecular half-life data comparable to ours, i.e. where predators were fed a single prey item. Whether by serological or PCR assay, half-lives for insect predators have not exceeded 20 h, while those for spiders tend to be much longer. The very long half-life we derived for P. maculiventris is hence more spider-like than insect-like, and leads one to wonder whether these sit-and-wait predators with sucking mouthparts may share some physiological adaptations, such as lower metabolic rates (Anderson, Reference Anderson1970; Greenstone & Bennett, Reference Greenstone and Bennett1980), with spiders, many of whom have a similar hunting style and feeding mode.
A lower resting metabolic rate would be an asset for a predator that is unable, or disinclined, to emigrate, enabling it to endure longer intervals between meals. Since such animals are apt to remain in the habitat longer, they would also epitomize one of the virtues of generalist predators: the ability to subsist on alternate prey, possibly at lower densities, until pests arrive (Symondson et al., Reference Symondson2002). The existence of a negative correlation between detectability half-life and resting metabolic rate is a hypothesis that can be tested when more data on both parameters are available.
The taxonomic breadth of both predators and prey for which half-lives have been determined is rather narrow (table 4). Comparable studies of more groups will enable us to identify some of the taxonomic and physiological correlates of the detectability half-life. This may lead to derivation of general principles that will assist us in the analysis of predator–prey relations, and the formulation of testable hypotheses on the relative importance of different predator groups as agents of biological control.
Published molecular half-lives of prey remains (sensuGreenstone & Hunt, Reference Greenstone and Hunt1993) in which each predator was fed a single prey item.

Acknowledgements
The authors thank Michael Athanas, Edward Clark, Jennifer Curtis and Lynda Liska for assistance with insect rearing; Robert Bennett for capturing Podisus; Richard Crosland for collecting L. haldemani; and Jon Lundgren and Natalia Vandenberg for observations on coccinellid feeding behaviour. This paper benefited greatly from comments by James Harwood, Robert O'Neill and Eric Riddick. The authors also thank the two anonymous reviewers for their comments.


