Introduction
Macroscopic Ediacaran fossils range from 579 to 541 Ma and are the oldest known large, architecturally complex biota in the fossil record (Narbonne, Reference Narbonne2011). Ediacara-type taxa consist of soft-bodied organisms preserved as casts or molds, typically at the bases of event beds induced by storms, turbidity currents, or volcanic eruptions. Preservational conditions characteristic of the Ediacaran sea floor, e.g., the prevalence of microbial mats and a lack of pervasive bioturbation (Gehling, 1999; Seilacher, Reference Seilacher1999), allowed for their preservation in numerous fossil localities around the world (Narbonne, Reference Narbonne2005; Fedonkin et al., Reference Fedonkin, Gehling, Grey, Narbonne and Vickers-Rich2007; Xiao and Laflamme, Reference Xiao and Laflamme2009; Erwin et al., Reference Erwin, Laflamme, Tweedt, Sperling, Pisani and Peterson2011). There has been a great deal of controversy surrounding the affinities of the Ediacara biota with a wide variety of interpretations. In general, however, focus has shifted from classifying the Ediacara biota as a whole to evaluating each Ediacaran taxon separately, and at present, the prevailing view is that many or most Ediacaran taxa represent extinct clades at a high taxonomic level along with some stem-group animals, including potential sponges and mollusks (Fedonkin et al., Reference Fedonkin, Gehling, Grey, Narbonne and Vickers-Rich2007; Xiao and Laflamme, Reference Xiao and Laflamme2009, Erwin et al., Reference Erwin, Laflamme, Tweedt, Sperling, Pisani and Peterson2011; Sperling et al., Reference Sperling, Peterson and Laflamme2011; Laflamme et al., Reference Laflamme, Darroch, Tweedt, Peterson and Erwin2013). Considerable controversy still exists for the affinities of many Ediacaran taxa.
Ediacaran fronds in particular were traditionally interpreted as pennatulacean cnidarians (e.g., Sprigg, Reference Sprigg1947, Reference Sprigg1949; Glaessner and Wade, Reference Glaessner and Wade1966; Anderson and Conway Morris, Reference Anderson and Conway Morris1982; Jenkins, Reference Jenkins1985, Reference Jenkins1992; Boynton and Ford, Reference Boynton and Ford1995) or ctenophores (Gürich, Reference Gürich1933; Dzik, Reference Dzik2002), but other interpretations have included fungi or fungi-grade organisms (Peterson et al., Reference Peterson, Waggoner and Hagadorn2003), elaborate colonies of prokaryotes (Steiner and Reitner, Reference Steiner and Reitner2001), terrestrial lichens (Retallack, Reference Retallack1994, Reference Retallack2013), or organisms belonging to an extinct high-level clade, either at the kingdom level (Seilacher, Reference Seilacher1992) or the phylum level within the Metazoa (Pflug, Reference Pflug1970, Reference Pflug1972; Buss and Seilacher, Reference Buss and Seilacher1994). Interpretations of Ediacaran fronds as cnidarian or ctenophore filter feeders have been discarded due to the absence of openings large enough to accommodate filter-feeding polyps or other feeding structures (Narbonne, Reference Narbonne2004). Interpretations that require photosynthesis have been discarded for all taxa found in Newfoundland on the basis of numerous sedimentological studies of the strata in which the fossils are found in that area, which conclude that the depositional environment was deep marine, well below the photic zone (Misra, Reference Misra1971; Myrow, Reference Myrow1995; Wood et al., Reference Wood, Dalrymple, Narbonne, Gehling and Clapham2003; Ichaso et al., Reference Ichaso, Dalrymple and Narbonne2007; Mason et al., Reference Mason, Narbonne, Dalrymple and O’Brien2013). Geochemical evidence is not consistent with a chemosynthesis-based ecosystem (Canfield et al., Reference Canfield, Poulton and Narbonne2007). The current leading hypothesis is that they are stem-group animals that represent an early ‘failed experiment’ in metazoan evolution (Narbonne, Reference Narbonne2005; Xiao and Laflamme, 2009; Liu et al., 2015). This interpretation is supported by paleoecological analyses (Clapham and Narbonne, Reference Clapham and Narbonne2002; Clapham et al., Reference Clapham, Narbonne and Gehling2003), which found that, in the census populations preserved in situ in the Mistaken Point area (Figs. 1, 2), the biota show epifaunal tiering and other ecological patterns similar to those observed in metazoan filter-feeding communities of the Phanerozoic (Narbonne, Reference Narbonne2005).
(1) Location map showing the study area in the southeast of the island of Newfoundland. The Avalon Terrane is in dark gray. (2) Geologic map of the Mistaken Point area, with the Mistaken Point E-surface marked with a star. The G-surface is exposed meters away from the E-surface. Adapted from Clapham et al., Reference Clapham, Narbonne and Gehling2003.

Ediacaran stratigraphy of the eastern Avalon Peninsula. The Mistaken Point E-surface is marked with a star. U–Pb dates from Benus (Reference Benus1988) and Narbonne et al. (Reference Narbonne, Xiao and Shields2012b). Fm.=Formation; Gp.=Group.
The Mistaken Point area is exceptional for its abundance and diversity of deep-marine Ediacaran fossils preserved beneath ash beds. The vast majority of taxa found there have been studied and described in great detail (e.g., Gehling and Narbonne, Reference Gehling and Narbonne2007; Laflamme et al., Reference Laflamme, Narbonne, Greentree and Anderson2007; Bamforth et al., Reference Bamforth, Narbonne and Anderson2008; Liu et al., Reference Liu, McIlroy, Antcliffe and Brasier2011, Reference Liu, Kenchington and Mitchell2015) and used in paleoecological studies (Clapham and Narbonne, Reference Clapham and Narbonne2002; Clapham et al., Reference Clapham, Narbonne and Gehling2003; Darroch et al., 2013). However, many of the stemmed, small-frond fossils have previously received relatively little attention, which this study seeks to redress.
Ediacaran frond morphology
The frond body plan is common among Ediacaran assemblages all over the world (Laflamme and Narbonne, Reference Laflamme and Narbonne2008b), including South Australia (Glaessner and Daily, Reference Glaessner and Daily1959; Jenkins and Gehling, Reference Jenkins and Gehling1978), Namibia (Pflug, Reference Pflug1970, Reference Pflug1972; Narbonne et al., Reference Narbonne, Saylor and Grotzinger1997; Vickers-Rich et al., Reference Vickers-Rich, Ivantsov, Trusler, Narbonne, Hall, Wilson, Greentree, Fedonkin, Elliott, Hoffmann and Schneider2013), the White Sea area of Russia (Fedonkin, Reference Fedonkin1985), central England (Boynton and Ford, Reference Boynton and Ford1995; Wilby et al., Reference Wilby, Carney and Howe2011), and eastern Newfoundland, Canada (Misra, Reference Misra1971; Narbonne and Gehling, Reference Narbonne and Gehling2003; Laflamme et al., Reference Laflamme, Narbonne and Anderson2004, 2007; Hofmann et al., Reference Hofmann, O’Brien and King2008; Narbonne et al., Reference Narbonne, Laflamme, Greentree and Trusler2009). This paper follows the morphological terminology proposed by Laflamme and Narbonne (Reference Laflamme and Narbonne2008a, Reference Laflamme and Narbonneb).
Ediacaran fronds are generally composed of three main parts (Fig. 3): a basal holdfast, typically bulbous or disc-shaped; a stem and/or central stalk (the stalk being an extension of the stem into the petalodium); and a leaf-like, morphologically complex petalodium (Laflamme and Narbonne, Reference Laflamme and Narbonne2008a, Reference Laflamme and Narbonneb), the ornamented leaf-like section generally composed of two or more ‘petaloids’ (Laflamme and Narbonne, Reference Laflamme and Narbonne2008a, Reference Laflamme and Narbonneb), each composed of repeating modules arranged in branches attached to the stalk or stem. The petalodium, as the most morphologically complex and variable part of the frond, is most important for identification and classification (Jenkins and Gehling, Reference Jenkins and Gehling1978). The largest branches connected directly to the stem or stalk are termed primary branches; any smaller branches that emerge from those branches are termed secondary branches, and even smaller branches attached to the secondary branches are termed tertiary branches. The frond body plan characteristic of many Ediacaran taxa is likely an example of convergent evolution due to shared ecology—in this case, a common need to elevate above the substrate, the same reason that frond-shaped morphologies are observed today across several kingdoms (plants, animals, and fungi; Laflamme and Narbonne, Reference Laflamme and Narbonne2008b). Laflamme and Narbonne (Reference Laflamme and Narbonne2008a, Reference Laflamme and Narbonneb) described four distinct branching architectures that they regarded as apomorphies for four high-level taxonomic groups within the Ediacara biota. Three of these are known from Mistaken Point: Arborea-type branching, which consists of parallel primary branches attached to a central stalk at right angles with teardrop-shaped secondary branches; Rangea-type branching, which has been called fractal—self-similar over at least three orders of magnitude, and constructed from individual ‘rangeomorph frondlets’; and Charnia-type branching, which is subcategory of Rangea-type, composed of sigmoidal primary branches with a zigzagging central axis, and secondary modular elements that are composed of tertiary rangeomorph elements. The latter two belong to a high-level clade called the Rangeomorpha (Pflug, Reference Pflug1972; Jenkins, Reference Jenkins1985; Narbonne, Reference Narbonne2004; Laflamme et al., Reference Laflamme, Darroch, Tweedt, Peterson and Erwin2013), and the first constitutes a clade called the Arboreomorpha (Laflamme et al., Reference Laflamme, Darroch, Tweedt, Peterson and Erwin2013). Rangeomorphs, along with the arboreomorph genus Charniodiscus Ford, Reference Ford1958, dominate the deep-sea Ediacaran assemblages of eastern Newfoundland (Narbonne, Reference Narbonne2004; Hofmann et al., Reference Hofmann, O’Brien and King2008; Narbonne et al., Reference Narbonne, Laflamme, Greentree and Trusler2009) and central England (Boynton and Ford, Reference Boynton and Ford1995; Wilby et al., Reference Wilby, Carney and Howe2011; Liu et al., 2015), and are known sparingly from younger and shallower Ediacaran localities (Fedonkin et al., Reference Fedonkin, Gehling, Grey, Narbonne and Vickers-Rich2007).
Generalized morphology of a stemmed frond. The three main components are the holdfast, stem, and the petalodium. Primary branches can be attached to a central stalk, as in the right half of the figure, or to the distal end of the stem, as in the left half of the figure.
Laflamme et al. (Reference Laflamme, Xiao and Kowalewski2009) concluded that Ediacaran fronds could have absorbed dissolved organic carbon osmotrophically, and that the fractal branching of rangeomorph elements would have increased surface-area-to-volume ratios sufficiently for this to be a viable strategy. This mode of feeding is used today mainly among bacteria, but a larger pool of available dissolved organic carbon in the Ediacaran combined with the high surface-area-to-volume ratio would have made this a viable feeding strategy for macroscopic Ediacaran organisms (Laflamme et al., Reference Laflamme, Xiao and Kowalewski2009). It is therefore suggested that the tiering observed in the rangeomorph-dominated assemblages in eastern Newfoundland and central England evolved due to competition to take maximum advantage of the dissolved organic carbon in the water column of their environments, and that this was the ecological pressure that led to the convergent evolution of a frond body plan among multiple clades in the Ediacaran (Laflamme and Narbonne, Reference Laflamme and Narbonne2008b).
Geological setting
Much of eastern Newfoundland, including the Avalon, Bonavista, and Burin peninsulas, is part of the Avalon Terrane (O’Brien et al., Reference O’Brien, Wardle and King1983; Myrow, Reference Myrow1995; Fig. 1.1), which consists of Neoproterozoic and early Paleozoic strata that were deposited on and adjacent to the microcontinent Avalonia, a volcanic arc off the coast of Gondwana (Nance et al., Reference Nance, Murphy and Keppie2002; Pisarevsky et al., Reference Pisarevsky, McCausland, Hodych, O’Brien, Tait and Murphy2011). Architecturally complex fossils have been found in three main locations in Ediacaran strata of the Avalon Terrane of eastern Newfoundland (Fig. 1): the Mistaken Point area on the southeastern tip of the Avalon Peninsula (see review by Narbonne et al., Reference Narbonne, Xiao and Shields2012b); the Spaniard’s Bay area in the northwest of the Avalon Peninsula (Narbonne, Reference Narbonne2004; Ichaso et al., Reference Ichaso, Dalrymple and Narbonne2007; Flude and Narbonne, Reference Flude and Narbonne2008; Narbonne et al., Reference Narbonne, Laflamme, Greentree and Trusler2009); and the Catalina Dome on the eastern coast of the Bonavista Peninsula (O’Brien and King, Reference O’Brien and King2004; Hofmann et al., Reference Hofmann, O’Brien and King2008; Mason et al., Reference Mason, Narbonne, Dalrymple and O’Brien2013). Ediacaran fossils occur commonly to abundantly in the Drook, Briscal, and Mistaken Point formations of the Conception Group, and the Trepassey and Fermeuse formations of the St. John’s Group (Fig. 1.1, 1.2). The small frond specimens included in this study were found in the Mistaken Point Formation in the Mistaken Point Ecological Reserve, Avalon Peninsula.
The Mistaken Point Formation is the uppermost formation in the Conception Group, part of a deep marine siliciclastic succession that overlies the mainly igneous rocks of the Harbour Main Group (King, Reference King1988, Reference King1990). The Mistaken Point Formation is dominated by mudstone-rich, siliciclastic turbidites deposited at the toe-of-slope in a forearc basin (Misra, Reference Misra1971; Wood et al., Reference Wood, Dalrymple, Narbonne, Gehling and Clapham2003; Ichaso et al., Reference Ichaso, Dalrymple and Narbonne2007; Mason et al., Reference Mason, Narbonne, Dalrymple and O’Brien2013). The turbidites are primarily Bouma T(C)DE beds (Bouma, Reference Bouma1962), with ‘TF’ interturbidite, laminated mudstone deposits from the low energy intervals between turbidity currents (e.g., Hesse, Reference Hesse1975; Wood et al., Reference Wood, Dalrymple, Narbonne, Gehling and Clapham2003). The absence of wave-generated structures or evidence of exposure in several kilometers of stacked turbidites in the succession implies that the depositional environment was at great depth, from which it has been inferred that organisms living in that environment could not have relied on photosynthesis (Wood et al., Reference Wood, Dalrymple, Narbonne, Gehling and Clapham2003; Narbonne, Reference Narbonne2005; Ichaso et al., Reference Ichaso, Dalrymple and Narbonne2007). In addition to the mudstone-rich siliciclastic turbidites, the succession is punctuated by thin beds of volcanic ash from the adjacent island arc deposited within the TF divisions, which are responsible for the preservation of the soft-bodied organisms beneath them (Seilacher, Reference Seilacher1999; Wood et al., Reference Wood, Dalrymple, Narbonne, Gehling and Clapham2003; Ichaso et al., Reference Ichaso, Dalrymple and Narbonne2007) in what Narbonne (Reference Narbonne2005) termed ‘Conception-style preservation.’ Because ash layers are less resistant than the silicified mudstone, the rocks tend to weather along the planes of ash beds and expose the surface of the mudstone immediately underneath. The fossils are preserved as both positive and negative epireliefs on these surfaces (Narbonne, Reference Narbonne2005). Frond-shaped organisms, which were tethered to the sea floor but otherwise were flexible in the water column, were typically oriented in a common direction with other fronds on the same rock surface, either parallel with the downslope direction inferred from Bouma TC-division turbidite current ripples or in a contour-parallel orientation 90° counterclockwise from the downslope direction (Wood et al., Reference Wood, Dalrymple, Narbonne, Gehling and Clapham2003).
The Mistaken Point assemblage
The Mistaken Point Ecological Reserve, southeastern Avalon Peninsula, Newfoundland, is famous for its exceptional Ediacaran fossils that are exposed on numerous broad, flat surfaces along the coastal cliffs (Misra, Reference Misra1971; Narbonne et al., Reference Narbonne, Gehling and Vickers-Rich2007). These surfaces are effectively snapshots of the Ediacaran sea floor, with fossils of the soft-bodied biota preserved in relief by episodic burial by volcanic ash. The succession (Fig. 2) contains many significant fossil horizons, including the oldest known complex macroscopic fossils, found in the Drook Formation (Narbonne and Gehling, Reference Narbonne and Gehling2003), dated at 578.8±0.5 Ma (van Kronendonk et al., Reference Van Kronendonk, Gehling and Shields2008; Narbonne et al., Reference Narbonne, Xiao and Shields2012b). These include the rangeomorph fronds Trepassia Narbonne, Laflamme, Greentree, and Trusler, Reference Narbonne, Laflamme, Greentree and Trusler2009 (see also Narbonne and Gehling, Reference Narbonne and Gehling2003); Charnia Ford, Reference Ford1958 (see also Laflamme et al., Reference Laflamme, Narbonne, Greentree and Anderson2007), and a possible specimen of Charniodiscus (see Liu et al., Reference Liu, McIlroy, Matthews and Brasier2012); along with the possible early sponge (Sperling et al., Reference Sperling, Peterson and Laflamme2011) Thectardis Clapham, Narbonne, Gehling, Greentree, and Anderson, Reference Clapham, Narbonne, Gehling, Greentree and Anderson2004. The oldest known stemmed fronds, Culmofrons Laflamme, Flude, and Narbonne, Reference Laflamme, Flude and Narbonne2012, are found in the overlying Briscal Formation, along with the branching rangeomorph Bradgatia Boynton and Ford, Reference Boynton and Ford1995 (see Flude and Narbonne, Reference Flude and Narbonne2008) and the spindle-shaped rangeomorph Fractofusus Gehling and Narbonne, Reference Gehling and Narbonne2007. Above that, the Mistaken Point Formation is the most richly fossiliferous part of the succession, with diverse assemblages of rangeomorphs and other Ediacaran taxa preserved at Gull Rock Cove and Mistaken Point itself (Clapham et al., Reference Clapham, Narbonne and Gehling2003; Wood et al., Reference Wood, Dalrymple, Narbonne, Gehling and Clapham2003), including the well-known and well-studied Mistaken Point E-surface, dated at 565±3 Ma (Benus, Reference Benus1988; Narbonne et al., Reference Narbonne, Xiao and Shields2012b), on which most of the fossils in this study are found. The overlying Trepassey Formation also contains fossil assemblages preserved by ash (Wood et al., Reference Wood, Dalrymple, Narbonne, Gehling and Clapham2003; Bamforth et al., Reference Bamforth, Narbonne and Anderson2008). Above that formation, ash deposition had ceased in this part of Newfoundland, so the taphonomic window allowing for preservation of architecturally complex Ediacaran fossils was closed (Gehling et al., Reference Gehling, Narbonne and Anderson2000; Wood et al., Reference Wood, Dalrymple, Narbonne, Gehling and Clapham2003; Narbonne, Reference Narbonne2005; Mason et al., Reference Mason, Narbonne, Dalrymple and O’Brien2013).
Over the last decade, numerous taxa have been described from the Mistaken Point area and the E-surface in particular, as well as elsewhere in the Ecological Reserve and elsewhere in Newfoundland. These have included taxa known from Charnwood Forest, England and new taxa, totaling 26 types (Narbonne et al., Reference Narbonne, Laflamme and Thomas2012a). Many of these taxa have been rangeomorphs: organisms constructed of numerous similar, fractally branching rangeomorph ‘modules’ assembled into a variety of different body plans (Narbonne, Reference Narbonne2004), e.g., the reclining, spindle-shaped Fractofusus (Gehling and Narbonne, Reference Gehling and Narbonne2007), comb-shaped Pectinifrons Bamforth, Narbonne, and Anderson, Reference Bamforth, Narbonne and Anderson2008, bush-shaped Bradgatia (Flude and Narbonne, Reference Flude and Narbonne2008), stemless elongate frond Charnia (Laflamme et al., Reference Laflamme, Narbonne, Greentree and Anderson2007), and the stemmed, tulip-shaped frond Culmofrons (Laflamme et al., Reference Laflamme, Flude and Narbonne2012). Mistaken Point taxa that do not belong to the Rangeomorpha include Thectardis (Clapham et al., Reference Clapham, Narbonne, Gehling, Greentree and Anderson2004) and the stemmed arboreomorph frond with a discoid holdfast Charniodiscus (Laflamme et al., Reference Laflamme, Narbonne and Anderson2004). All known taxa were benthic and immobile, although Liu et al. (Reference Liu, McIlroy and Brasier2010) reported a single level of putative trace fossils implying surficial locomotion from Mistaken Point.
Virtually all fossils in the Mistaken Point area have been named, with the notable exception of many of the small fronds. Many small fronds are simply juveniles of known taxa; Liu et al. (Reference Liu, McIlroy, Matthews and Brasier2012) reported the discovery of particularly tiny juvenile fronds from the Drook Formation, most of which can be identified as Charnia, Trepassia, or possibly Charniodiscus. However, some small fronds exist in the Mistaken Point Formation that bear little resemblance to any named taxa. Hofmann et al. (Reference Hofmann, O’Brien and King2008) described two distinctive small frond taxa from the Bonavista Peninsula—Primocandelabrum Hofmann, O’Brien, and King, Reference Hofmann, O’Brien and King2008 and Parviscopa Hofmann, O’Brien, and King, Reference Hofmann, O’Brien and King2008—which bear no resemblance to any larger Ediacaran taxa. In previous paleoecological work at Mistaken Point (Clapham and Narbonne, Reference Clapham and Narbonne2002; Clapham et al., Reference Clapham, Narbonne and Gehling2003), many small, stemmed fronds were grouped together and informally called ‘dusters,’ but closer inspection finds significant disparity within that informal grouping, including representatives of the taxon Primocandelabrum from the Bonavista Peninsula.
Interpretation of the small fronds has been problematic due to taphonomy. Because of the mode of preservation of the Mistaken Point biota, the resolution of the fossils is dependent upon the grain size of the ash beneath which they are preserved. This mode of preservation presents a problem for the study of the smallest fossils in the assemblage in particular, because their features are often obscured proportionally more than in larger specimens. Other Ediacaran fronds are classified heavily on the basis of their secondary and tertiary branching, which are not discernible in most small frond specimens. Because of this difficulty, the small fronds are some of the last fossils of the Mistaken Point E-surface to be described systematically, and only the best-preserved specimens can be identified with confidence.
Methods
Removal of fossils from the Mistaken Point Ecological Reserve is strictly prohibited, so paleontological study of the Mistaken Point biota relies heavily on field photographs, latex molds, and casts of the original fossils. A 70-m2 cast of the Mistaken Point E-surface was made by Research Casting International in 2009 and 2010 in association with the provincial government of Newfoundland and Labrador, the Royal Ontario Museum, Johnson GeoCentre, Queen’s University, and the University of Oxford. The complete cast is located in Research Casting International’s facility in Trenton, Ontario, and this was an invaluable resource because it allowed thorough inspection of a large portion of the Mistaken Point E-surface—on which most of the small frond fossils included in this study are found—in a controlled indoor environment. Two hundred and fifty-one fossils were numbered and photographed from this cast, although many were too poorly preserved and ambiguous to be identified in this study. Additional field photographs were taken in Newfoundland of small fronds on parts of the E-surface that were not included in the casting project, as well as of two fossils from the G-surface. Dozens of latex molds of these and other fossils made by the authors and other Queen’s University researchers were also used as resources and photographed for comparison. One original specimen (ROM 38641) that was previously collected from the E-surface by the Royal Ontario Museum was also included in this study.
Strata in the Mistaken Point area have been subjected to tectonic shortening of ~40% on most of the fossiliferous surfaces. This deformation is especially apparent in fossils with originally circular features, e.g., frond holdfasts, which are circular in every undeformed Ediacaran assemblage in the world (Ford, Reference Ford1958; Jenkins and Gehling, Reference Jenkins and Gehling1978; Boynton and Ford, Reference Boynton and Ford1995; Wilby et al., Reference Wilby, Carney and Howe2011). In the Mistaken Point area, these fossils have become oblong, all in the same direction and the same amount on a given bedding surface, elongate in the direction of cleavage (Seilacher, Reference Seilacher1999; Wood et al., Reference Wood, Dalrymple, Narbonne, Gehling and Clapham2003). To account for this deformation, each photograph was retrodeformed (i.e., stretched in the direction of shortening until oblong holdfasts became circular; Seilacher, Reference Seilacher1999; Wood et al., Reference Wood, Dalrymple, Narbonne, Gehling and Clapham2003; Ichaso et al., Reference Ichaso, Dalrymple and Narbonne2007). In specimens without a holdfast to use as a direct indicator of the degree of shortening, an average retrodeformational ratio from across the surface was used.
Once retrodeformed, each specimen was measured for a variety of dimensions: holdfast diameter, stem length, stem width, petalodium length, petalodium width, frond length, and basal petalodium angle. Ratios between these measurements were compared to find morphometric differences in overall shape of the fronds. Petalodium branching architecture was also carefully observed in sufficiently well-preserved specimens.
Approximately 270 fossils in total were numbered and photographed. Many were identified as or tentatively assigned to known Ediacaran taxa, including Charnia, Culmofrons, Bradgatia, Charniodiscus, Avalofractus Narbonne, Laflamme, Greentree, and Trusler, Reference Narbonne, Laflamme, Greentree and Trusler2009, Beothukis Brasier and Antcliffe, Reference Brasier and Antcliffe2009, and Primocandelabrum. Others were too ambiguous to identify as either existing taxa or newly defined taxa. For many potential small frond fossils from the E-surface, only the holdfast and stem/stalk were preserved, with no evidence of the petalodium.
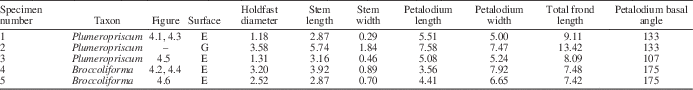
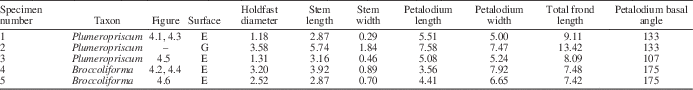
In all, five clear, well-preserved small fronds were determined to belong to two new monotypic genera. Measurements of these specimens are summarized in Table 1. Other small frond specimens with similar shapes might belong to these taxa, but due to poor preservation, such identifications are uncertain.
Measurements of retrodeformed specimens of Plumeropriscum and Broccoliforma. All measurements in centimeters except petalodium basal angle, which is measured in degrees.
Systematic paleontology
Group Rangeomorpha Pflug, Reference Pflug1972
Genus Plumeropriscum new genus
2003 ‘Feather dusters,’ Reference Wood, Dalrymple, Narbonne, Gehling and ClaphamWood et al., fig. 9.
2005 ‘Feather dusters,’ Reference NarbonneNarbonne, fig. 5e.
Type species
Plumeropriscum hofmanni n. sp., by monotypy.
Diagnosis
As per species.
Etymology
From the Spanish ‘plumero’ meaning feather duster, and the Latin ‘priscum’ meaning old.
Plumeropriscum hofmanni new species
Figures 4.1, 4.3, 4.5, 5.1, 5.2
Light photographs of new small frond taxa. (1) Unretrodeformed holotype fossil of Plumeropriscum hofmanni n. gen. n. sp. from the Mistaken Point E-surface. (2) Unretrodeformed holotype fossil of Broccoliforma alta n. gen. n. sp. from the Mistaken Point E-surface. (3) Retrodeformed latex mold of the holotype of Plumeropriscum hofmanni n. gen. n. sp.; white arrow points to a primary branch with visible secondary branching. (4) Retrodeformed latex mold of the holotype of Broccoliforma alta n. gen. n. sp. (5) Retrodeformed field photograph of an additional specimen of Plumeropriscum hofmanni n. gen. n. sp. on the Mistaken Point E-surface. (6) Retrodeformed photograph of an additional specimen of Broccoliforma alta n. gen. n. sp. from the E-surface cast at the Research Casting International facility in Trenton, Ontario. Scale bars=2 cm.
(1) Retrodeformed field photograph of the holotype of Plumeropriscum hofmanni n. gen., n. sp. (2) Sketch of the holotype of Plumeropriscum hofmanni n. gen. n. sp. based on numerous photographs of the fossil and latex molds under different lighting conditions. Secondary branching is visible in different areas of the fossil in different photographs depending on the light source. (3) Retrodeformed field photograph of the holotype of Broccoliforma alta n. gen. n. sp. (4) Sketch of the holotype of Broccoliforma alta n. gen. n. sp., based on numerous photographs of the fossil and latex molds. Scale bars=2 cm.
Holotype
On the Mistaken Point E-surface. Plastotype on the E-surface cast at the Royal Ontario Museum, ROM 60065.1.
Diagnosis
Cm-scale frondose fossil with a roughly deltoid petalodium attached to a bulbous or discoidal holdfast by a cylindrical stem. The petalodium consists of at least nine thin primary branches attached at the base of the petalodium extending upward distally from the base of the petalodium. Where well-preserved, rangeomorph architecture is subtly visible. No axial stalk is evident. Branches in the foreground can be seen in their entirety, but background branches are partially obscured beneath foreground branches, implying a bushy, mop-like shape of the organism before compaction.
Description
The holotype (Figs. 4.1, 4.3, 5.1, 5.2), from the Mistaken Point E-surface, is a 9.1 cm-long frond with a small, bulbous holdfast, 1.2 cm in diameter, attached to a cylindrical stem (2.9 cm long, 3 mm thick). At the end of the stem, many (at least 12 visible in this specimen), thin (1 mm or less) primary branches emerge from the base of the petalodium, forming a deltoid petalodium (5.5 cm long, 5 cm wide) with a 133° angle at the base, and an 80° angle at a pointed tip on the distal end of the petalodium. Additional primary branches emerge from behind the branches, with visible connections to the base. Subtle secondary branching is visible on several branches, which implies rangeomorph affinity.
In addition to the holotype, there are two more specimens that are well-preserved (Fig. 4.5): one also from the E-surface and the other from the slightly stratigraphically higher G-surface. Several other small frond fossils from Mistaken Point might belong to the species but are not preserved clearly enough to be certain. The G-surface specimen is somewhat larger than the two E-surface specimens, with a total length of 13.4 cm. Its holdfast, with a diameter of 3.5 cm, is also larger relative to its size. It is also the specimen of Plumeropriscum hofmanni n. gen., n. sp. with the least number (9) of visible primary branches. However, it does have a very similar shape and overall morphology to the holotype. The third specimen is very similar to the holotype, only with a slightly shorter stem and a more acute basal petalodium angle (107°), unlike the other two specimens with angles of 133°. Both of the additional specimens are somewhat more rounded than the pointed, deltoid holotype. Secondary branching is not visible on either.
Etymology
Named for the late Hans Hofmann who contributed greatly to our understanding of Ediacaran paleontology.
Comparisons
Plumeropriscum is similar to Primocandelabrum in that all of the primary branches are connected to the stem at the base of the petalodium. However, the branches of Plumeropriscum are thinner and more numerous, and the petalodium shape is more deltoid with a point at the distal end, compared to the inverse triangle shape of Primocandelabrum. The branches of Primocandelabrum are arranged as a two-dimensional fan as opposed to the three-dimensional, mop-like shape of Plumeropriscum.
The petalodium of Plumeropriscum has some similarities to Bradgatia in that there are many primary branches all attached together at the base, but Bradgatia lacks the stem and holdfast of Plumeropriscum and shows a great deal more secondary and tertiary branching that forms individual ‘petals’ in a way that Plumeropriscum does not.
An as yet unnamed stemmed frond from the Ediacaran deposits of Charnwood Forest, central England, informally referred to as the ‘dumbbell-like frond’ (Wilby et al., Reference Wilby, Carney and Howe2011), shows some similarity to Plumeropriscum, with an orbicular petalodium attached to a stem with a holdfast. However, the dumbbell frond’s holdfast is quite distinct from the small bulbous holdfast of Plumeropriscum; it is a large disc, larger even than the frond’s petalodium, with many concentric rings. Within the dumbbell frond’s petalodium, the branching pattern appears somewhat similar to that of Plumeropriscum, with no defined central axis and multiple primary branches attached at the base of the petalodium, but beyond that, the branching appears more complex in the dumbbell frond. It could be a closely related taxon.
Remarks
The three-dimensional, mop-like architecture of Plumeropriscum makes it unique among the Mistaken Point biota. The ‘mop’ of primary branches that make up the petalodium would likely have been an effective means of straining flowing water for nutrients in a different but analogous way to other fronds.
Group uncertain
Genus Broccoliforma new genus
Type species
Broccoliforma alta n.sp., by monotypy.
Diagnosis
As per species.
Etymology
From the Italian ‘broccolo’ referring to the vegetable, and the Latin ‘formis’ meaning shape.
Broccoliforma alta new species
Holotype
On the Mistaken Point E-surface. Plastotype at the Royal Ontario Museum, ROM 62623.
Diagnosis
Irregularly lobate, flabellate frond connected to a short cylindrical stem that attaches at the opposite end to a disk. Internal features consist of poorly developed lobes radiating in a semicircular, fan-shaped array from the center of the diameter, with an angle at the base of the petalodium near 180°.
Etymology
From the Latin ‘altus’ meaning deep, referring to the deep marine environment of the organism.
Description
The holotype (Figs. 4.2, 4.4, 5.3, 5.4), from the Mistaken Point E-surface, is a flabellate frond characterized by a large, bulbous holdfast (3.2 cm diameter), stem (3.9 cm long, 0.9 cm wide), and a roughly semicircular (3.5 cm long, 7.9 cm wide) petalodium. The flabellate petalodium has a sharp outer margin, and internal features of the petalodium consist of irregular, poorly developed lobes radiating in a fan-shaped array from the base of the petalodium where it attaches to the stem. The angle at the base of the petalodium is 175°, close to a horizontal line, and the petalodium itself is wider than it is long. Compared to other fronds, the holdfast, which appears as a thickened bulb continuous with the stem at its base, is notably large relative to the total length of the frond.
The other known specimen of Broccoliforma alta n. gen., n. sp. (Fig. 4.6), also from the E-surface, is slightly smaller but overall quite similar to the holotype. It also has a relatively large holdfast (2.5 cm), and thick stem (2.9 cm long, 0.4 cm wide). This specimen has similar overall petalodium morphology to the holotype, including the flabellate shape with a 175° angle of the base of the petalodium, and greater petalodium width than length (4.4 cm long, 6.7 cm wide).
Comparisons
In contrast to most other fronds (with the exception of some Primocandelabrum), the petalodium of Broccoliforma is wider than long. Its petalodium has the widest basal angle of any Mistaken Point stemmed organism. Similar to a number of other Ediacaran fronds, including Plumeropriscum as well as Avalofractus, Culmofrons, and Primocandelabrum, Broccoliforma has a round, bulbous holdfast and a cylindrical stem. The stem is somewhat thick compared to that of other small fronds, and the diameter of the holdfast is relatively large compared to the total length. Unlike other Mistaken Point fronds, the petalodium of Broccoliforma does not exhibit modular construction or branching that is apparent even in poorly preserved frond fossils of a similar size. Instead, Broccoliforma has an irregular lobate morphology. Given the rough, radiating geometry of the lobes and the wide petalodium, it is possible that Broccoliforma is a taphomorph of Primocandelabrum in which the branches are not clearly preserved but other structures are, but until more specimens are found this is difficult to resolve.
The lobate structure of the petalodium bears a resemblance to other lobate fossils from the Mistaken Point biota known as ivesheadiomorphs (Liu et al., Reference Liu, McIlroy, Antcliffe and Brasier2011), a group that includes the genera Ivesheadia Boynton and Ford, Reference Boynton and Ford1995 (see also Boynton and Ford, Reference Boynton and Ford1996), and Blackbrookia Boynton and Ford, Reference Boynton and Ford1995, although Liu et al. (Reference Liu, McIlroy, Antcliffe and Brasier2011) regarded all ivesheadopmorphs as taphomorphs of other taxa and therefore as variants of each other. The somewhat oblong shape and raised perimeter of the petalodium of the holotype are particularly reminiscent of the taxon Blackbrookia, which is primarily known from Charnwood Forest, England (Boynton and Ford, Reference Boynton and Ford1995; Wilby et al., Reference Wilby, Carney and Howe2011) and is also reported from Bonavista Peninsula (Hofmann et al., Reference Hofmann, O’Brien and King2008). The frond morphology of Broccoliforma, in contrast with the irregular, unstructured shapes of Blackbrookia and Ivesheadia, could be useful in interpreting other lobate Ediacaran taxa.
Remarks
The lobate, irregular Ivesheadiomorpha (Boynton and Ford, Reference Boynton and Ford1995; Liu et al., Reference Liu, McIlroy, Antcliffe and Brasier2011) is a controversial group of taxa from the Ediacaran biota of eastern Newfoundland and Charnwood Forest. When Boynton and Ford first described them in 1995, they interpreted them as cnidarian-grade organisms, but this view has fallen out of favor. Three alternative explanations have recently been put forward: Laflamme et al. (Reference Laflamme, Schiffbauer and Narbonne2011) suggested that they are microbial colonies; Liu et al. (Reference Liu, McIlroy, Antcliffe and Brasier2011) argued that they are taphomorphs of other Ediacaran taxa representing advanced stages of decay; and Wilby et al. (Reference Wilby, Carney and Howe2011) put forward the idea that they are the result of upright fronds causing sediment deposition beneath them during turbidity current flow.
Unfortunately, none of these explanations for ivesheadiomorphs can be used to interpret Broccoliforma. If the morphological similarity between Broccoliforma and Blackbrookia is homologous, the existence of a stem and holdfast attached to the lobate structure is inconsistent with the microbial interpretation of Laflamme et al. (Reference Laflamme, Schiffbauer and Narbonne2011) or the sediment deposition explanation of Wilby et al. (Reference Wilby, Carney and Howe2011), which respectively require a simpler morphology, and an accumulation of sediment beneath an elevated frond’s petalodium, not at the end of the stem of a horizontally felled frond. Similarly, the flabellate shape of the Broccoliforma is unique among Mistaken Point fronds, making it difficult to reconcile as a taphonomic degradation of some more common Mistaken Point frond as inferred for Ivesheadia by Liu et al. (Reference Liu, McIlroy, Antcliffe and Brasier2011). An alternative explanation is to echo the original interpretation of Boynton and Ford (Reference Boynton and Ford1995) that ivesheadiomorphs are tissue-grade organisms themselves, albeit apparently lacking any of the apomorphies of the Cnidaria. This interpretation would suggest that perhaps another clade of Ediacaran organisms evolved convergently into a frondose body plan in order to extend higher into the water column to compete for nutrients.
Other small fronds at Mistaken Point
Apart from these two newly described small fronds, there are several other taxa that share a broadly similar morphology and that would have occupied the same ecological tier at Mistaken Point. These include juveniles of larger fronds present on the surface (i.e., Charnia, Charniodiscus, and Beothukis), as well as taxa only known as small fronds from elsewhere in eastern Newfoundland: Primocandelabrum (Fig. 6.2) from the Bonavista Peninsula (Hofmann et al. Reference Hofmann, O’Brien and King2008), and Avalofractus (Fig. 6.1) from Spaniard’s Bay. Some might be juveniles of the recently described Culmofrons, which is found lower in the succession in the Mistaken Point area (Laflamme et al., Reference Laflamme, Flude and Narbonne2012). Many of the fossils that Clapham and Narbonne (Reference Clapham and Narbonne2002) and Clapham et al. (Reference Clapham, Narbonne and Gehling2003) referred to as ‘dusters’ are now known to be Primocandelabrum or Beothukis, whereas others could be juvenile Culmofrons.
(1) Avalofractus from the Mistaken Point E-surface. White arrow points to a primary branch that shows secondary branching. (2) Primocandelabrum from the Mistaken Point E-surface. White arrow points to a primary branch that shows subtle secondary branching. (3) Large frond from the E-surface at Watern Cove; this fossil has a similar shape to other fossils identified as Primocandelabrum, but the two thick secondary branches are unique. Scale bars=2 cm.
Primocandelabrum is a stemmed frond with a petalodium shaped like an inverted triangle constructed by a few thick primary branches attached at the base of the petalodium. It was first described from the Mistaken Point and Trepassey formations of the Bonavista Peninsula (Hofmann et al., Reference Hofmann, O’Brien and King2008). Hofmann et al. (Reference Hofmann, O’Brien and King2008, p. 212) proposed that many of the small fronds at Mistaken Point represent specimens of Primocandelabrum sp. but did not illustrate or cite any specific specimens attributed to this taxon. The tentaculate holdfast of the species Primocandelabrum hiemaloranum Hofmann, O’Brien, and King, Reference Hofmann, O’Brien and King2008 has not been observed at Mistaken Point, but one specimen from the Mistaken Point E-surface shows subtle secondary branches attached to its thick primary branches, suggesting rangeomorph architecture (Fig. 6.2). On the Mistaken Point E-surface at Watern Cove, there is a large frond that resembles Primocandelabrum (Fig. 6.3) with two thick primary branches attached at the base of the petalodium, but uniquely to this specimen, each of these branches also has a thick secondary branch attached that points inward toward the central axis at an ~60° angle. The total length of the frond is 12.7 cm, with a particularly wide petalodium, measuring 5.6 cm long and 12.3 cm wide. This specimen might be a separate species of Primocandelabrum, or considering its greater size than most Primocandelabrum, perhaps a more mature specimen.
Beothukis has a spatulate shape that in some specimens makes it appear as if it might have a stem between the holdfast and the petalodium, which allows for confusion with the true Plumeropriscum ‘dusters,’ especially in specimens that are small and poorly preserved. Other stemmed small fronds on the Mistaken Point E-surface bear a resemblance to Culmofrons from Lower Mistaken Point and the Briscal Formation, but they are not sufficiently well-preserved to classify them definitively to this genus. Juvenile Charnia and Charniodiscus fronds also share this low tier.
Discussion
When Clapham and Narbonne (Reference Clapham and Narbonne2002) and Clapham et al. (Reference Clapham, Narbonne and Gehling2003) first studied the paleoecology of Mistaken Point, many of the taxa included in their analysis were still undescribed and unnamed, but most, such as the ‘spindle’ (now called Fractofusus) and the ‘pectinate’ (now called Pectinifrons), were nonetheless readily discernible due to their unique constructions. However, the smaller taxa were more problematic when approached informally, and a wide variety of small frond fossils that share a broadly similar organism-scale shape were grouped together as ‘dusters,’ including these two new taxa, Plumeropriscum and Broccoliforma, as well as the relatively recently described Primocandelabrum, Beothukis, Avalofractus, and Culmofrons.
Consequently, it is worth noting that the lower tier occupied by the small fronds has more diversity than previously realized in paleoecological analysis. At Mistaken Point, there are a number of different small fronds, many of which are not known as larger taxa, and most of which have a broadly similar overall body shape. Small fronds from the E-surface show significant overlap in terms of stem length versus total frond length, and petalodium length versus width (Fig. 7). This observation is in contrast with Spaniard’s Bay, where the various types of small fronds are distinct from each other based on the same criteria (Narbonne et al., Reference Narbonne, Laflamme, Greentree and Trusler2009). The Spaniard’s Bay types plot into three distinct groups, whereas the Mistaken Point taxa show significant overlap, which makes differentiating and identifying the numerous poorly preserved specimens challenging. Primocandelabrum in particular has a large morphometric range that both Plumeropriscum and Broccoliforma fall within, although their unique constructions allow them to be differentiated. Although there is not great disparity in the overall shape of the small, stemmed fronds, there is considerable diversity in petalodium architecture. It can therefore be concluded that this tier was a competitive one, with significant convergent evolution of multiple taxa.
Comparison of the morphometric distribution of Mistaken Point small, stemmed fronds with the small fronds described by Narbonne et al. (Reference Narbonne, Laflamme, Greentree and Trusler2009) in the Spaniard’s Bay area. Distribution of Mistaken Point taxa on the chart is represented by empty ellipses; distribution of Spaniard’s Bay taxa is represented by patterned ellipses. Mistaken Point taxa show significantly more overlap, meaning that the overall body shape of the fronds shows convergence across multiple frond architectures.
In addition to the small fronds that were lumped together as ‘dusters,’ other, less similar taxa also share the same tier, slightly elevated from the substrate, adding to its biodiversity. These taxa include the bush-like rangeomorph Bradgatia (Flude and Narbonne, Reference Flude and Narbonne2008), the triangular potential sponge Thectardis (Clapham et al., Reference Clapham, Narbonne, Gehling, Greentree and Anderson2004; Sperling et al., 2011), and the comb-like rangeomorph Pectinifrons (Bamforth et al., Reference Bamforth, Narbonne and Anderson2008), as well as juveniles of taxa such as Charniodiscus and Charnia.
Conclusions
Although the small frond fossils of Mistaken Point are difficult to interpret and to identify due to the limitations of their taphonomy and overall similarity in first-order shape, two new taxa have been described on the basis of their unique petalodium constructions: the mop-like Plumeropriscum hofmanni n. gen., n. sp., and lobate, flabellate Broccoliforma alta n. gen., n. sp.
With description of the small frond fossils previously informally referred to together as ‘dusters,’ the last major gap in the taxonomic description of the known Mistaken Point assemblage is filled, excluding fossils that are currently too unclear and poorly preserved to describe meaningfully. Future discoveries of similar fossils with better preservation in Newfoundland, England, or elsewhere, could shed light on remaining unnamed fossils at Mistaken Point, and on the two taxa described in this study based on a small number of specimens with suboptimal preservation. Now that the decade-long endeavor to describe all of the major fossils of the Mistaken Point assemblage is essentially complete, it could be enlightening to revisit detailed paleoecological study of the Mistaken Point biota, keeping in mind the greater taxonomic disparity and competition now known to have existed at this tier of the ecosystem.
Acknowledgments
Narbonne acknowledges funding from the Natural Sciences and Engineering Research Council of Canada (NSERC) and a Queen’s University Research Chair. Mason acknowledges scholarship funding from NSERC, and the Ontario Ministry of Training, Colleges, and Universities, and Queen’s University. C. Carbone’s assistance in the field was invaluable to this study. T. Boag and R. Abrams are thanked for their assistance with fossil and latex photography; A. Mann is thanked for illustrating the two new small frond taxa, and C.L. Wilson is thanked for her assistance in creating the names. Fieldwork in the Mistaken Point Ecological Reserve was carried out under scientific permits granted by the Parks and Natural Areas Division, Government of Newfoundland and Labrador. Research Casting International in Trenton, Ontario is thanked for providing access to the Mistaken Point E-surface cast. We also thank the people of Portugal Cove South and Trepassey, Newfoundland for their kindness and hospitality during our field work. P. Vickers-Rich and S. Xiao are thanked for their helpful reviews of this manuscript.