


1. Introduction
There is a deep and persisting tension that exists between the conception(s) of time in modern physics and philosophy and the conception of time that seems to stem naturally from human first-person phenomenological experience. As time is presented to us in experience, it seems to have a character that intrinsically involves dynamicism and change. That is, based on phenomenology alone, it has appeared plausible to many to conclude that temporality involves something that might be characterized as “spatiotemporal perspective-independent change” in regard to what is true about reality. The coherence of this notion of perspective-independent change (which I will refer to henceforth as “real” change) is known, however, to come into serious question fairly quickly both upon philosophical reflection as well as upon attempts at successful scientific theorizing.
John Ellis McTaggart (Reference McTaggart1908) famously illustrated one powerful line of reasoning that leads to skepticism about real change by adopting a spatiotemporal ontology of events. McTaggart demonstrated that if one takes real change to mean that these events change in their properties of being past, present, or future, then one is inevitably led to require an infinite regress of additional metatemporal dimensions in order to make sense of these changing properties. Albert Einstein’s Special and General Theories of Relativity, being the dominant and most empirically well-confirmed theories within modern spacetime physics, are also generally taken to threaten the possibility of real change. This is due to the facts that time within these theories is conceived of as one dimension within a four-dimensional manifold and that the geometrical structure of this manifold does not allow for absolute facts regarding simultaneity.
These considerations, among others, have led many to embrace what has been referred to as the block universe view, in which all events can be assigned a four-dimensional coordinate (three spatial coordinates, x, y, and z, and one temporal coordinate, t) and reality just consists of all of these events timelessly existing within the resulting four-dimensional space (or manifold). In the block view, there is no real change, because what event exists at any point in the manifold permanently exists at that point in a frozen and unchanging way, and there is nothing that singles out any points within the temporal or spatial dimensions of the manifold as being any more real than any others.
If the block-theorist wishes to defend her view against those who maintain that time is metaphysically dynamic, a proper accounting of why the world would seem dynamic to us despite the fact that it is not appears to be required, and many such attempts have been made. One approach, in broad strokes, has been to attempt to ground asymmetries in our psychological experiences of past, present, and future in more basic physical asymmetries regarding the laws of nature or the distribution of matter throughout the spacetime block.
More narrowly, several approaches have focused on what many physicists feel to be the most basic observed physical asymmetry, that of entropy (Hawking Reference Hawking, Halliwell, Pérez-Mercader and Zurek1994; Albert Reference Albert2003; Schulman Reference Schulman2005). The “entropic arrow of time” refers to the fact that, in modern physical theory, the entropy of a system appears to evolve through time asymmetrically such that it always increases toward the future and decreases toward the past. Entropy has appeared special with regard to this apparent temporal asymmetry due to the fact that within classical physics all of the dynamical laws appear to be time-symmetric. That is, if the laws of physics allow a process to occur in one direction, then they will also in principle allow this process to occur in reverse. Beyond the initial problem regarding the lack of real change within a block universe, then, there is a further problem in understanding why a universe with time-symmetric laws would seem to have many physical and psychological processes that only occur in one temporal direction but not the other. The statistical mechanical considerations pioneered by Ludwig Boltzmann are regarded by many as the solution to the problem of how time-symmetric laws can result in the empirically observed temporal asymmetry regarding entropic processes.
In 1877, Boltzmann characterized entropy with the following equation:
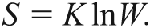
In this equation k is simply a constant and W is the number of microstates that are consistent with the current macrostate of the system in question. Entropy is therefore taken as a simple measure of how many different rearrangements one could perform on the microstates of a system without changing the macrostate. The more possible rearrangements, the higher the entropy. Boltzmann’s explanation for the entropic asymmetry, then, was simply one regarding probability. If one begins in a macrostate with very few possible rearrangements, then it is much more probable that the system in question will randomly evolve into a macrostate with more possible rearrangements.
Because Boltzmann’s statistical mechanical probabilities underpinning the entropic asymmetry are also time-symmetric, however, it has appeared to many that Boltzmann’s program could only be completed with additional assumptions. The reason for this is that if one happens to observe a low entropy state, Boltzmann’s framework actually implies that the probability is extremely high that one should reach a higher entropy state if the system is evolved either forward or backward in time. This has led to the suggestion of a “past hypothesis,” which asserts that the universe (or at least our part of it) began in a state of extremely low entropy. From Boltzmann’s statistical considerations, it would follow from this assumption that the probability of subsequent states of the universe having increasingly large entropy is extremely high. Further, without assuming such a low entropy boundary condition, Boltzmann’s reasoning could be taken to suggest that the ordered world we see around us, including our memories of the past, are more likely a random fluctuation out of a disordered, higher-entropy past state. Therefore, the past hypothesis has been further motivated by a desire to avoid a sort of global skepticism with regard to the accuracy of our memories. It has also been employed more specifically in attempts to explain the asymmetry we observe with regard to our psychological experience. David Albert (Reference Albert2003), for example, has attempted to demonstrate that the assumption of a past hypothesis, in conjunction with Boltzmann’s framework, is actually required for the formation of reliable “records” of past events and that this therefore explains why human brains contain memories of the past and not the future. The plausibility of the past hypothesis has also been challenged, however. John Earman (Reference Earman2006) has argued, for example, that there are serious problems that arise when one attempts to provide a measure of the Boltzmann entropy for the universe as a whole, and further that, even if this problem was overcome, it would not necessarily tell us much about why entropy increases are observed within the local subsystems within the universe that thermodynamics is usually concerned with.
Regardless of the truth of the past hypothesis, however, the success of statistical mechanics and the fact that locally observed systems always evolve toward high entropy states are both well confirmed empirically, and one can simply appeal to these noncontroversial facts regarding entropic asymmetries in such systems in an attempt to explain our temporal experience. To do so, one generally assumes that certain psychological processes must in some way depend on the entropy gradient observed within these types of systems. For example, one might assert that memories (or “records”) within a brain or other computational system could only compile in the direction of increasing entropy. If this were true, then a case might be made for why we have the psychological asymmetries that we do in regard to temporal experience. That is, if one were to randomly survey the perspective of the “me” existing at any spacetime point within the block universe, that “me” would have evidence of past events in his brain but no evidence of future events. Hence, he would have reason to believe that the past and the future from his perspective had different metaphysical status despite the fact that this was false (Horwich Reference Horwich1987).
One recent attempt to make just this move has been taken independently by Stephen W. Hawking and L. S. Schulman (Hawking Reference Hawking, Halliwell, Pérez-Mercader and Zurek1994; Schulman Reference Schulman2005). Under this attempt, an analogy is made between the human brain and modern computers, and it is then asserted that computational processes in computers (such as storing something in a computer’s memory) require that entropy is increasing. The claim is that whenever a computer stores something new in memory, the total entropy of the world always increases during such a process if one considers the heat given off by the process and so forth. So, to quote Hawking: “Thus computers remember things in the direction of time in which entropy increases. In a universe in which entropy is decreasing in time, computer memories will work backward” (Hawking Reference Hawking, Halliwell, Pérez-Mercader and Zurek1994, 348).
Schulman more explicitly relies on a principle demonstrated by Rolf Landauer (Reference Landauer1961) to make the same basic point. Landauer’s principle is claimed to show formally that memory in a computer could only work in the direction of increasing entropy. Schulman then claims that if such a computer were allowed a psychology, no asymmetry independent of the entropic arrow would be necessary to account for its asymmetrical experience of time.
In a recent paper, however, Owen J. E. Maroney (Reference Maroney2010, 28) has argued in detail against Schulman and Hawking. He concludes:
Any sequence of logical operations in an entropy increasing universe is physically possible in an entropy decreasing universe. Landauer’s Principle, as it is commonly stated, assumes statistical mechanical principles that are equivalent to being in an entropy increasing universe. If one changes those assumptions, so that one is in an entropy decreasing universe, a critical inequality in Landauer’s Principle in reversed. The physical implementation of logical operations, which increase entropy, do so, not by virtue of any inherent properties of the logical operation, but by virtue of being in an entropy increasing universe. If the same logical operation is performed in an entropy decreasing universe, it is entropy decreasing. As a result, entropy decreasing universes are not inherently hostile to the acquisition, persistence or utilization of information.
If Maroney is correct, then there is nothing intrinsic to logical operations in computers that requires entropy to be changing in any particular direction, and thus a computational arrow of time based on entropic considerations does not succeed. Maroney follows this conclusion, however, with the following remark: “If the psychological arrow of time is to be aligned with the thermodynamic arrow, it cannot be through the information processing properties of the brain. It may be through the biochemical structures that arise in Non-Equilibrium Steady State processes, but if so, it is certainly not through any information processing characterization of such structures” (Maroney Reference Maroney2010, 29).
Maroney’s closing remark then may be taken to suggest that if one is still interested in finding an entropic explanation for asymmetries in psychological experience, then one would need to look at aspects of the brain processes underlying psychological experience that do not fall under an abstract information-processing characterization. One may instead need to look to the unique implementation of these processes. This article seeks to further investigate the tenability of this possibility.
2. Entropic Considerations in Biological Processes
One paradigm case for illustrating the entropic asymmetry is that of diffusion. For example, if I have a container with a high concentration of energetic gaseous particles connected to a container with a lower concentration, then the statistical mechanical considerations underlying the entropic arrow make it extremely more likely that the future state will be one in which the concentrations in the connected containers become equal (i.e., a process of diffusion will occur where particles will flow from high to low concentration regions). Similarly, if I introduce a drop of red dye into a clear aqueous solution, entropic reasoning dictates that the dye particles will not remain in a concentrated clump but instead spontaneously diffuse equally throughout the aqueous medium. As a more quantitative illustration, consider two connected containers containing a total of 20 particles. Now consider the probability and entropy associated with a “nondiffused” state in which there are 15 particles in the left container and 5 in the right. To figure this out, we must first calculate W within Boltzmann’s equation above. The formula for W is
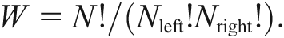
Following this formula for the 15left/5right configuration, we get 15,504 possible particle arrangements consistent with this macrostate. As there are 220 different possible arrangements of the 20 particles in total, the probability of the 15left/5right configuration comes out to roughly 1.5%, and if we enter in our calculated value for W into Boltzmann’s equation above, we get an entropy of  . Now we can compare this with the probability and entropy associated with a “diffused” state of 10 particles in each container. Performing the same calculations for a 10left/10right configuration, we get W = 184,756, the probability for this configuration comes out to roughly 18%, and
 . Thus, we can see that the entropy and probability associated with the diffused macrostate is higher than for the nondiffused state, and this lesson generalizes such that it is highly likely from these probabilistic considerations alone that, given low-entropy, nondiffused starting conditions, any system will evolve into the more diffused, higher-entropy state.
What is important to realize here is that if entropy within biological systems was not reliably increasing, or if we happened to live in a universe where entropy instead reliably decreased in the forward-time direction, then processes like diffusion would not reliably occur. In a world where entropy tended to stay the same, for example, our two connected containers would just remain in their state of unequal gas concentration, and in a world where entropy decreased, particle positions would evolve toward greater concentration inequalities.
These considerations are relevant precisely because it is a well-known fact that such diffusion/equilibration tendencies are heavily depended upon by many biological processes, including those thought to underlie computation and memory in the human and animal brain. As an illustration, I will briefly consider three such processes: synaptic transmission, gene expression, and action potential propagation (Byrne and Roberts Reference Byrne and Roberts2009).
Synaptic transmission is the means by which the voltage across the membrane in one neuron can influence the voltage across the membrane in another neuron it is synaptically connected with. Upon the arrival of an electrochemical signal, termed an action potential, neurotransmitter (NT) molecules are released from the presynaptic terminal of the sending neuron in order to cross a small space (the synapse) and bind to protein receptors on the receiving neuron. NT molecules influence these receptors in such a way as to affect an eventual change in voltage in the receiving cell. This transmission process depends upon diffusion/equilibration in three locations. First, when an action potential arrives to initiate NT release, it does so by opening calcium permeable membrane channels. Due to the existence of a calcium concentration gradient across the cell membrane, and the tendency for entropy to increase, calcium reliably diffuses into the cell and triggers the release of NT. Second, when NT is released, it does so from a small membrane-bound region of high NT concentration (called a vesicle), and its entropy-dependent tendency to diffuse to areas of low concentration across the synapse is necessary for it to reach its target receptors on the receiving cell. Third, effects of NT on the receiving cell typically involve opening membrane channels permeable to electrically charged ions. These ions flow into the receiving neuron and affect its voltage level due to an ion concentration gradient similar to that described for calcium above.
A major computation that neurons are thought to perform by this process is the summing of positive and negative electrical potentials (in the form of ions diffusing in and out of the cell from multiple active synapses).The neurons receiving these local voltage changes subsequently initiate output signals only when the sum is above a certain voltage threshold. It should be clear that the implementation of this summing computation, as well as the synaptic processes that lead to it, would not work without spontaneous diffusion, and hence without the assumption of increasing entropy.
Gene expression is a process in which a copy of part of the genetic code in DNA travels out of a cellular nucleus in the form of a similar molecule called mRNA and is then used to inform a protein called a ribosome regarding the sequence of amino acids to link together in order to create a specific functional protein. This process relies on the newly created mRNA leaving a region of high mRNA concentration in the nucleus and diffusing out of the nucleus to come into contact with the ribosome in a region of lower mRNA concentration. If mRNA tended to remain concentrated in the nucleus (as would be the case under an assumption of stable or decreasing entropy), then the process of gene expression would not work and could not work in reverse. Empirical work has demonstrated that long-term memory formation is dependent upon gene expression in certain brain regions such that if gene expression is blocked, then memory formation fails (Lynch Reference Lynch2004). Thus, memory formation is known to depend on cellular processes, which themselves depend on spontaneous diffusion and hence on increasing entropy.
Action potential propagation is the process by which electrochemical signals are transmitted down the axon of a neuron in order to trigger NT release onto its target cells. An action potential is essentially a traveling wave of sodium ion diffusion into an axon followed by potassium ion diffusion out of an axon, and it also depends on stable concentration gradients of these ions. If the concentration gradients of sodium and potassium across the cell membrane are not maintained, then action potentials will not travel. Thus, this phenomenon also depends on diffusion being a reliably spontaneous process. It should be noted, however, that while in the case of NT release and gene expression diffusion is the primary driving force, in the case of ionic diffusion, considerations of electrostatic pressure also play a role.
These three examples do not exhaust all of the neural processes that depend on an assumption of increasing entropy, but they should be sufficient to make the point. If ions and molecules did not reliably move from regions of high concentration to regions of lower concentration due to spontaneous diffusion, then (1) a neuron would not be able to sum together positive and negative inputs to compute an output, (2) a neuron would not be able to transmit that output toward a synapse, and (3) the signal would not transmit across a synapse. Further, there is both theoretical and empirical support for the notion that memory formation and maintenance in the brain involves stable changes in the strengths of the effects of synaptic activity on receiving neurons and that this process depends on gene expression as well as other diffusion-dependent cellular processes (Lynch Reference Lynch2004). As mentioned above, if one chemically blocks gene expression, then one can reliably interrupt memory formation in experimental animals.
Given this information, it appears plausible to argue that since spontaneous diffusion in the forward-time direction is a defining feature of an entropy-increasing universe, and since processes critical to successful brain function and memory formation (including, but not limited to, synaptic transmission and gene expression) depend critically on passive diffusion being a reliable and spontaneous process, successful brain function and memory formation also depend on increasing entropy in the forward-time direction. From this conclusion, one could also infer that memory formation in biological brains could not occur without spontaneous diffusion, and hence could not occur in the forward-time direction within a universe where entropy either decreased or remained stable in the forward-time direction of that universe.
If this argument is sound, then a novel solution to the discrepancy between temporal experience and the block universe view presents itself naturally. If it is sound, that is, we can now begin again by assuming a block universe with time-symmetric laws in which every event at every spacetime coordinate is equally real and in which there is no moving present, then we can simply ask what that universe should feel like to a biological brain that exists at any one of those spacetime coordinates. If that universe contained a past-future asymmetry in its matter distribution such that entropy always increased in the future direction for biological brain-like systems, then, according to the argument above, any biological brain at any spacetime coordinate would only have been able to compile its spontaneous diffusion-dependent memories in the past-to-future direction, and hence it would only have knowledge of facts regarding past moments. Thus, any biological brain we survey, at any of the “equally real and existing” spacetime coordinates within this block universe, will only be able to compile memories in this future direction, will thus only have reason to believe that events in its past have occurred, and hence will feel as though future and past moments relative to its position in the block universe have a different metaphysical status.
Notice that this explanation simply depends on the fact that, since biological systems are believed to have arisen spontaneously, they must rely on at least some spontaneous processes, and entropic reasoning is one major contributor in determining which processes are and are not spontaneous in a given universe. This entropic reasoning regarding the spontaneity of a given process will then ultimately depend on whether entropy increases, decreases, or remains constant in a given direction through time for local systems within that universe. Notice also that this explanation relies entirely on contingent facts about the biochemical implementation of the computational processes that occur within biological brains in a way that is fully independent of their abstract information processing description. Hence Maroney’s argument against Hawking’s and Schulman’s attempts to provide a thermodynamic arrow of time to computers should not apply to this proposal. Even if a computer’s memories (abstractly characterized in terms of information processing) could in principle compile in a direction of decreasing entropy, a biological brain’s memories cannot, and this is for reason’s entirely contingent on the implementation mechanisms that biology has had available to it over evolutionary time. As the dynamics of biological processes depend significantly upon diffusion-based dynamics within aqueous systems, for our purposes, we can capture the essence of what is required for intra- and intercellular communication processes with a simple model, such as a miniature goldfish bowl filled with water and a drop of red dye. Imagine that I insert a drop of red dye into any location within this goldfish bowl and that for “successful biological signaling” one of these dye molecules must reliably reach a detector within a random location on a distant edge of the bowl within a reasonable amount of time. In an entropy-increasing universe, the spontaneous diffusion process makes the probability of one of these dye molecules randomly bumping into this detector high as they spread to evenly fill the aqueous volume of the bowl. However, an entropy-decreasing universe would imply that the dye molecules would evolve toward being increasingly concentrated in a single region instead (i.e., the time reverse of diffusion), effectively ruling out any reasonable possibility of successful biological signaling and communication within our model.
It is important to note that this is a significantly weaker and more specific claim than what has been sought after previously. The claim here is simply that biological brains produce temporally asymmetric psychologies because they contingently happen to depend on certain physical implementation processes and not others. It is not the strong claim sought after previously to show that any information processing could only occur in one temporal direction. Thus the proposal of this article leaves open the possibility that functionally equivalent brain-like systems that made use of a different physical implementation system might experience time differently. It is also important to note that all asymmetric percepts may not be adequately accounted for by this proposal. Here I have argued that an entropy-based neurological asymmetry could give rise to an asymmetry in information processing and memory formation, and I have then appealed to the view that having memories of the past and not the future could influence one’s temporal phenomenology (Horwich Reference Horwich1987). It is not clear, however, that such an asymmetry can fully account for all dynamical aspects of perception, such as, for example, percepts of motion, which plausibly involve more than just asymmetries. Therefore, the present proposal only aims to illustrate a plausible account of how entropic asymmetries may relate to psychological asymmetries by means of their neurobiological implementation, and it does not claim to fully account for all dynamic aspects of phenomenology by means of highlighting this connection.
3. Conclusion
To conclude, then, the argument of this article is simply that human psychological functions (including memory formation) depend upon successful biological signaling, and hence such psychological functions are temporally asymmetric precisely because the biological signaling asymmetries that underlie them depend critically upon entropic asymmetries. We happen to find ourselves within a universe that is temporally asymmetric with respect to its entropic distribution of matter throughout spacetime, and hence we can only compile memories and perform other psychological functions in one temporal direction. According to this account, however, this temporal asymmetry within our minds/brains is merely an artifact of the contingent physical implementation our brains happen to use to perform computations, consistent with the fact that abstractly considered information-processing systems may in principle be physically implementable within universes that decrease in entropy instead. Finally, as the major arguments of this article depend only on empirically confirmed aspects of biological signaling and the entropic behavior of local systems, the present thesis also avoids controversial issues regarding the validity of a “past hypothesis” that threaten other major accounts of temporal asymmetries within human psychological experience.


