Introduction
Invasive organisms can have major impacts on the environments they invade. They have an effect on biodiversity and are one of the main causes of extinction (Diamond, Reference Diamond1989; Courchamp et al., Reference Courchamp, Chapuis and Pascal2003; Raven & Yeates, Reference Raven and Yeates2007). They can also deeply affect communities and change ecosystem processes (e.g. Atkinson & Cameron, Reference Atkinson and Cameron1993; Lonsdale, Reference Lonsdale1999; Mack et al., Reference Mack, Simberloff, Lonsdale, Evans, Clout and Bazzaz2000; Levine et al., Reference Levine, Vila, D'antonio, Dukes, Grigulis and Lavorel2003; Sanders et al., Reference Sanders, Gotelli, Heller and Gordon2003). Due to increased human movement and climate change, the prevalence of invasive organisms is likely to increase in the future (Hobbs & Mooney, Reference Hobbs, Mooney, Mooney, Mack, Mcneely, Neville, Schei and Waage2005).
Knowledge of the biology, natural history and biological requirements of a given invasive organism is valuable in order to facilitate management and control, and to predict potential distribution. For example, information on genetic variation and reproductive mode of a species can contribute to predicting its longer-term impacts. Due to a typically small number of individuals initially introduced, many invaders experience bottlenecks due to low genetic variation in the introduced population (Lambrinos, Reference Lambrinos2004). Invasive organisms may undergo rapid evolution to adapt to local conditions, although this is more likely if genetic variation is high for evolution to act upon (Lee, Reference Lee2002; Kawecki & Ebert, Reference Kawecki and Ebert2004). Furthermore, genetic variation can affect the capacity to colonize and invade (Tagg et al., Reference Tagg, Innes and Doncaster2005; Crawford & Whitney, Reference Crawford and Whitney2010) and thus has important implications in terms of the success of invaders (Roman & Darling, Reference Roman and Darling2007; Lucek et al., Reference Lucek, Roy, Bezault, Sivasundar and Seehausen2010).
Invasive organisms sometimes shift from sexual reproduction to obligate or facultative parthenogenesis in their invasive range (e.g. Moran, Reference Moran1992; Dybdahl & Lively, Reference Dybdahl and Lively1995; Sunnucks et al., Reference Sunnucks, England, Taylor and Hales1996). Without any need for mating, parthenogenesis allows populations to increase quickly, with a two-fold reproductive advantage compared to sexual populations (Maynard Smith, Reference Maynard Smith1978). Although rapid increase in population size is an advantage for parthenogens, genotypic variation may be very low; and, in the absence of genetic recombination, natural selection is unable to act on individual genes or chromosomal regions. In situ adaptation, therefore, may be considered less likely. Thus, the success of parthenogenetic invasive organisms has been attributed mainly to phenotypic plasticity or to the introduction of different specialized asexual genotypes (Peccoud et al., Reference Peccoud, Figueroa, Silva, Ramirez, Mieuzet, Bonhomme, Stoeckel, Plantegenest and Simon2008). Nonetheless, evolution by mutation can occur and lead to new phenotypes of ecological significance (Lynch, Reference Lynch1985; Sunnucks et al., Reference Sunnucks, Chisholm, Turak and Hales1998; Loxdale, Reference Loxdale2008).
There are different types of parthenogenesis, with different consequences for population genotypic variation. Automictic parthenogenesis involves meiosis and, therefore, the possibility of recombination (so daughters differ genetically from their mothers), although some forms result in increasing and high homozygosity. In apomictic parthenogenesis, new forms or clones can occur only following mutation and chromosomal rearrangements, and so daughters are genotypically very similar to their mother (Suomalainen, Reference Suomalainen1962). Genotypic variation is generally expected to be low in apomictic parthenogenesis, although this depends on rates of formation of new asexual lineages from sexual ancestors, population sizes and mutation rates (Loxdale, Reference Loxdale2008, Reference Loxdale, Schön, Martens and Dijk2009). In many parthenogens, individuals capable of sexual reproduction can also be produced.
Molecular tools have revolutionized our understanding of population biology and ecology. Of all the genetic markers available, high resolution microsatellite markers are by far the most commonly used in ecological studies (Selkoe & Toonen, Reference Selkoe and Toonen2006). Microsatellites or simple sequence repeats (SSRs) are repeated motifs of one to six bases found mainly in the non-coding areas of the genome and have several favourable properties as genetic markers (Sunnucks, Reference Sunnucks2000). They are typically selectively neutral and highly length-variable (Chambers & MacAvoy, Reference Chambers and MacAvoy2000), and this polymorphism makes them very applicable to focus on fine-scale questions that were previously impossible to tackle (Zane et al., Reference Zane, Bargelloni and Patarnello2002; Selkoe & Toonen, Reference Selkoe and Toonen2006). For example, their variability makes them ideal for distinguishing individual genotypes and assessing levels of gene flow between populations (Lowe et al., Reference Lowe, Harris and Ashton2004). They are also well suited for assessing mating strategies and reproductive modes. For example, sexual and asexual populations are readily distinguished (e.g. Gómez & Carvalho, Reference Gómez and Carvalho2000; Wilson et al., Reference Wilson, Sunnucks, Blackman and Hales2002; Vorburger et al., Reference Vorburger, Lancaster and Sunnucks2003).
The willow sawfly, Nematus oligospilus (Hymenoptera: Tenthredinidae), is native to North America (southern Alaska to Mexico) and Eurasia (Ireland to the Himalayas), where it is widespread (Smith, Reference Smith, Krombein, Hurd, Smith and Burks1979), whilst it has been introduced into Argentina (Dapoto & Giganti, Reference Dapoto and Giganti1994), South Africa (Urban & Eardley, Reference Urban and Eardley1995), New Zealand (Berry, Reference Berry1997; Charles et al., Reference Charles, Allan and Fung1998) and Australia (Bruzzese & McFadyen Reference Bruzzese and McFadyen2006; Ede et al., Reference Ede, Caron and Clements2007). It has spread quickly after each new introduction (Dapoto & Giganti, Reference Dapoto and Giganti1994; Urban & Eardley, Reference Urban and Eardley1995; Cowie, Reference Cowie2006; Caron, Reference Caron2011). Population densities can increase rapidly, resulting in defoliation of willow trees and substantial damage in some areas (Cowie, Reference Cowie2006; Ede et al., Reference Ede, Hunt, Clements and Caron2009). On the basis of natural history data such as only females being observed, N. oligospilus is thought to be parthenogenetic in its invasive range, whereas both sexes occur in the native range (Charles et al., Reference Charles, Allan and Fung1998; Koch & Smith, Reference Koch and Smith2000). However, rare and unobserved sexual reproduction is common in parthenogens (Hurst et al., Reference Hurst, Hamilton and Ladle1992). If it can be established that it is indeed parthenogenetic in its invaded range, N. oligospilus provides an opportunity to study the ongoing ecology and evolution of an invasive species that has lost sexual reproduction. Effective molecular markers are necessary to establish the reproductive mode, spread and population dynamics of N. oligospilus.
Like all Hymenoptera, the ancestral reproductive mode for tenthredinid sawflies is haplodiploidy (arrhenotoky); females are the product of fertilization and have two copies of each chromosome, whilst males arise from unfertilized eggs and carry only a maternal haploid set of chromosomes (Normark, Reference Normark2003). Parthenogenesis occurs in many species and is obligate in some (Craig & Mopper, Reference Craig, Mopper, Wagner and Raffa1993). In some insects, males are unknown (Benson, Reference Benson1950), while in others, a few males are produced and their role is ambiguous (Craig & Mopper, Reference Craig, Mopper, Wagner and Raffa1993). Both apomictic and automictic parthenogenesis occur in tenthredinids (Suomalainen, Reference Suomalainen1962; Knerer, Reference Knerer, Wagner and Raffa1993).
Tenthredinid sawflies have been relatively little studied compared to other groups of Hymenoptera. Nonetheless, due to interesting life characteristics, such as their reproductive mode and feeding strategies, and because tenthredinids have undergone recent evolutionary radiation, they can be studied in order to investigate ecological and evolutionary theories concerning host-plant relationships, trophic interactions, speciation and adaptive radiation (Knerer, Reference Knerer, Wagner and Raffa1993; Roininen et al., Reference Roininen, Price and Tahvanainen1996; Price et al., Reference Price, Roininen and Ohgushi2005; Nyman et al., Reference Nyman, Farrell, Zinovjev and Vikberg2006a, 2010). However, little has so far been done on population biology and mating systems of this group taking advantage of highly-resolving molecular markers such as microsatellites. Previous population studies on phylogeography have used allozymes (Müller et al., Reference Müller, Barker, Boeve, De Jong, De Vos and Brakefield2004), while studies into heritability of defence traits were conducted using laboratory crosses (Müller et al., Reference Müller, Zwaan, De Vos and Brakefield2003). Most other molecular genetic studies on this group have used mitochondrial DNA (Nyman et al., Reference Nyman, Farrell, Zinovjev and Vikberg2006a, Reference Nyman, Vikberg, Smith and Boevé2010; MacQuarrie et al., Reference MacQuarrie, Langor and Sperling2007). Microsatellites developed for N. oligospilus could also prove useful for other sawfly species, although microsatellites developed from one species are typically less likely to be useful in genetically more distant species. Success of cross-amplification depends on the group targeted (e.g. Primmer et al., Reference Primmer, Møller and Ellegren1996; Zane et al., Reference Zane, Bargelloni and Patarnello2002; Zenger et al., Reference Zenger, Eldridge, Pope and Cooper2003; Wilson et al., Reference Wilson, Massonnet, Simon, Prunier-Leterme, Dolatti, Llewellyn, Figueroa, Ramirez, Blackman, Estoup and Sunnucks2004; Barbarà et al., Reference Barbarà, Palma-Silva, Paggi, Bered, Fay and Lexer2007; Palma-Silva et al., Reference Palma-Silva, Cavallari, Barbará, Lexer, Gimenes, Bered and Bodanese-Zanetti2007).
The aims of the present study were twofold. The first was to determine the reproductive mode of N. oligospilus with the level of asexual (clonal) diversity by developing and applying microsatellite markers. Since sawflies represent an interesting study group, the second aim was to assess the applicability of the microsatellites so designed in different sawfly species of varying relatedness to N. oligospilus.
Materials and methods
Study organisms
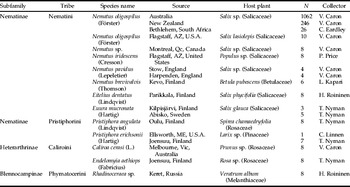
Nematus oligospilus individuals from different parts of the invasive range were used for the study. Individuals originated from South Africa, the North and South Island of New Zealand, and from eastern and western Australia. Although widespread, N. oligospilus is inconspicuous in its native range (Pschorn-Walcher, Reference Pschorn-Walcher and Schwenke1982). Individuals thought likely to be N. oligospilus were collected from Arizona, USA from sites where previous studies have been performed on this species (Carr et al., Reference Carr, Roininen and Price1998) and in Montreal, Canada at a specific site where several specimens preserved in insect collections originated (V. Caron, personal observation). Other species chosen for this study, such as Nematus brevivalvis Thomson, were closely related to N. oligospilus as shown in previous studies (Nyman et al., Reference Nyman, Vikberg, Smith and Boevé2010), while some other species were less closely related, belonging to other nematine tribes (e.g. Pristiphora spp.) and other subfamilies (e.g. Caliroa cerasi L., Rhadinoceraea sp. and Endelomyia aethiops F.; table 1).
Sawfly species used in this study with the source, host plant, collector and number of individuals used (N)

The tenthredinid species assessed here encompassed different life strategies. Some are gall-formers such as Euura mucronata Hartig (Nyman, Reference Nyman2002). Pristiphora angulata Lindqvist is a facultative miner of flower buds, while the others are external feeders. Many are parthenogenetic, including C. cerasi, E. aethiops and Pristiphora erichsonii Hartig (Benson, Reference Benson1950). Species like N. pavidus and Nematus iridescens Cresson are gregarious; the other species tested are primarily solitary but can occur at high population densities, as seen in N. oligospilus in its invasive range (Ede, Reference Ede2009). Many of the species chosen in this study are economically important. For example, C. cerasi (pear or cherry slug) can cause important damage to fruit trees (Carl, Reference Carl1972) and has been accidentally introduced to several countries including New Zealand and Australia (Naumann et al., Reference Naumann, Williams and Schmidt2002). Similarly, P. erichsonii, commonly known as the larch sawfly, can become a destructive pest of larch Larix sp. (Boévé, Reference Boévé and Capinera2004).
Microsatellite development
DNA was extracted using the 2 × CTAB extraction protocol (Grosberg et al., Reference Grosberg, Levitan and Cameron1996) from legs of four N. oligospilus individuals collected from different areas in Australia and preserved in 96% ethanol. Microsatellite loci were developed using the FIASCO enrichment protocol (Zane et al., Reference Zane, Bargelloni and Patarnello2002) with minor alterations. The initial digestion did not contain Bovine Serum Albumin (BSA) and the pre-amplified product was cleaned with 0.1 volume of 3M NaOAc and 2.5 volume of 100% ethanol, followed by an overnight incubation at –20 °C. The product was then centrifuged at 13,200 rpm (Centrifuge 5415D, Eppendorf, Hamburg, Germany) for 30 min and 70% ethanol washed. The DNA pellet was resuspended in 30 μl of 1 × TE. After cleaning, 400 ng of the pre-amplified PCR product was hybridized to two probes, (AC)17 and (ATT)17, which were then captured with Streptavidin MagneSphere Paramagnetic Particles (Promega, Madison, WI, USA) as described in Roberts & Weeks (Reference Roberts and Weeks2009). PCR products amplified from the enriched DNA pool were cloned using a TOPO TA Cloning Kit for Sequencing according to the manufacturer's instructions (Invitrogen). Eighty-seven clones were commercially sequenced (Macrogen Inc., Seoul, Korea).
DNA extraction for microsatellite screening
Between 250 and 1300 N. oligospilus individuals, most at the larval stage, were tested for each microsatellite locus, while six to ten individuals of each of the other sawfly species were screened. DNA was extracted from individuals preserved in 96% ethanol using the salting-out DNA extraction protocol described in Sunnucks & Hales (Reference Sunnucks and Hales1996). DNA pellets were re-suspended in 50 to 100 μl of 1 × TE buffer.
Microsatellite screening
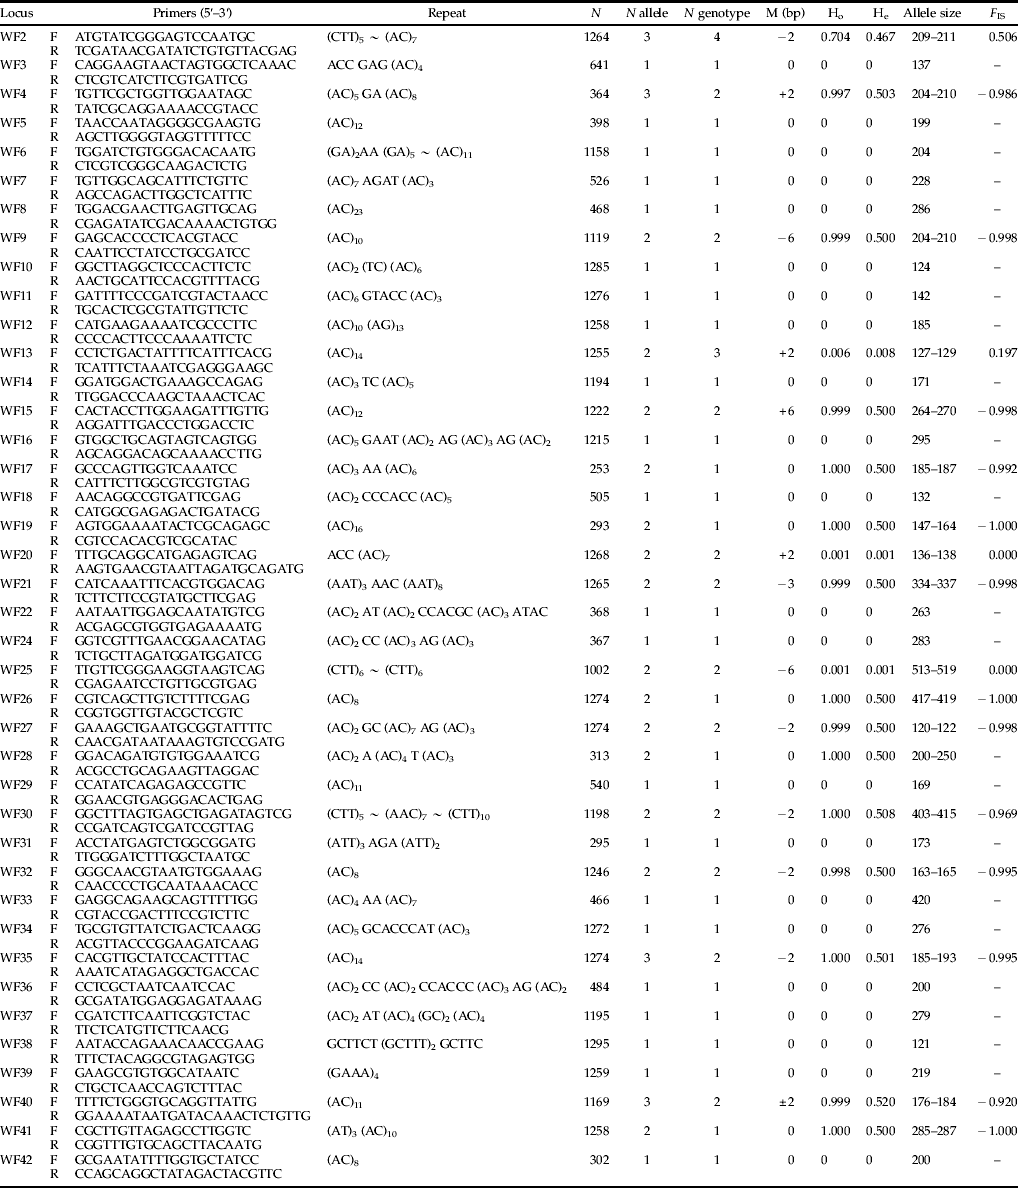
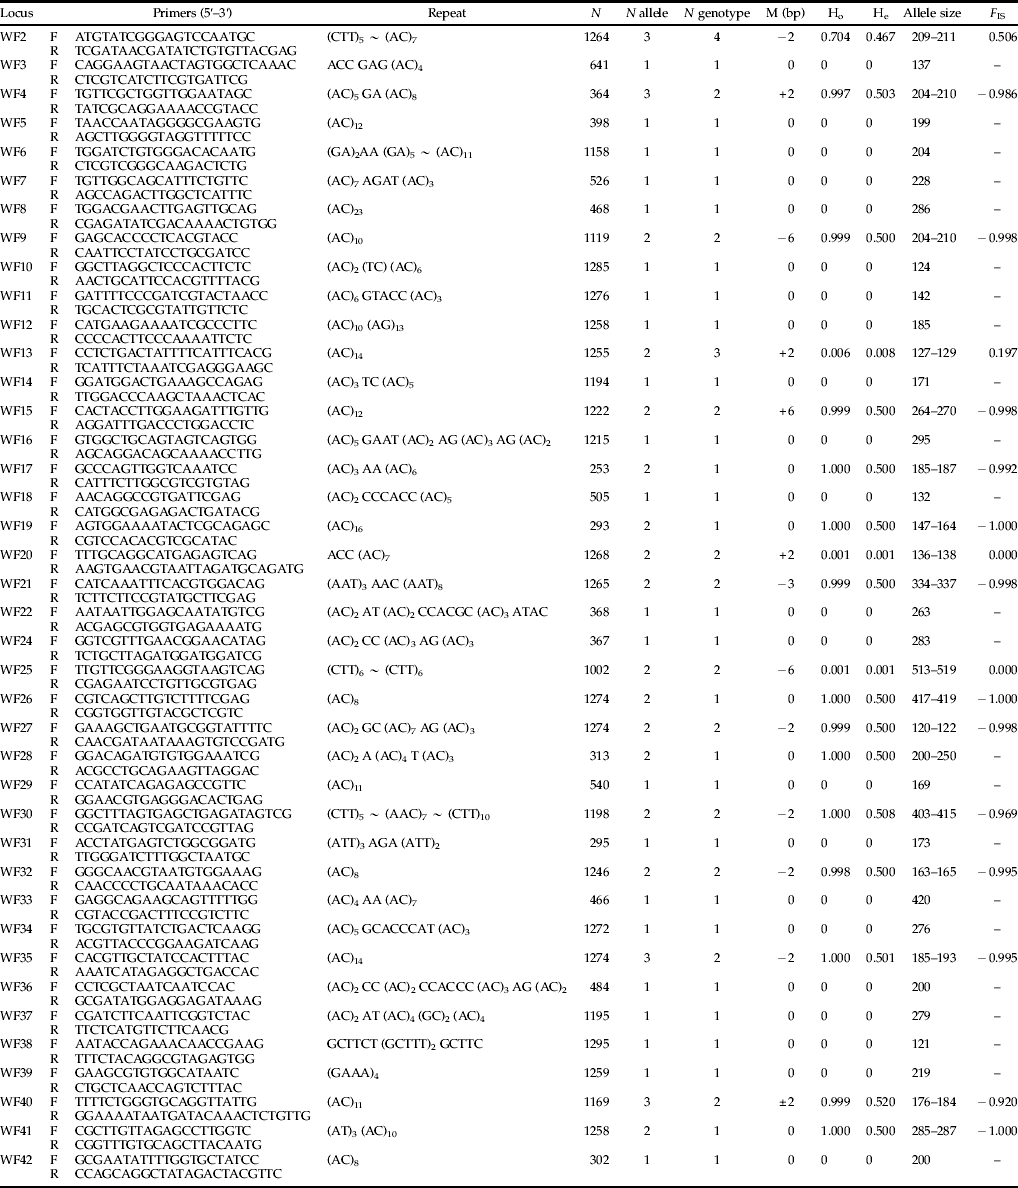
Following sequencing of DNA clones enriched for microsatellites, 43 primer pairs were designed using Primer3 v.0.4.0. (Rozen & Skaletsky, Reference Rozen, Skaletsky, Krawetz and Misener2000) (table 2). One primer of each pair was labelled with infra-red dyes IRD™700 or IRD™800 (LI-COR Biosciences, Lincoln, NE, USA). PCR reactions contained: 1 μl of 10×Taq buffer, 0.8 μl of 25 mM MgCl2, 1.6 μl of 1.25 mM dNTPs, 0.5 μl of 10 mg ml−1 BSA, 0.4 μl of Taq Polymerase (Fermentas, Burlington, Canada), 0.5 μl of 1 μM of each primer, 0.3 μl of 1 μM of IRD™700 or IRD™800, 1 μl of DNA template and Milli-Q water for a total volume of 10 μl. Cycling conditions were: 94 °C for 4 min, 35 cycles of 94 °C for 1 min, 55 °C for 30 s, 72 °C for 1 min, with the annealing temperature of the first five cycles reducing by 1 °C per cycle, the remaining 30 cycles having an annealing temperature of 50 °C, all followed by a final extension of 72 °C for 5 min. Multiplex reactions were prepared using the Qiagen PCR multiplexing kit (Qiagen, Hilden, Germany) when possible, to a maximum of 13 loci per PCR, following the manufacturer's instructions. PCR products were electrophoresed with LI-COR Global IR2 two-dye DNA sequencers (models 4200 and 4300).
Characteristics of microsatellite loci isolated from Nematus oligospilus. Locus name, primer sequence, core repeat in sequenced clone, number of individuals tested (N), number of alleles, number of genotypes, number of base pairs lost or gained when compared to main genotype (M), observed (Ho) and expected (He) heterozygosity, range of allele size, and F IS
Mitochondrial DNA (mtDNA) analysis
To estimate genetic similarities within N. oligospilus and among species, Cytochrome oxidase I mtDNA was sequenced using primers HCO1490 and LCO2198 (Folmer et al., Reference Folmer, Black, Hoeh, Lutz and Vrijenhoek1994). Seventy-four N. oligospilus individuals were assayed from 18 sites (14 in Australia, three from New Zealand, one from South Africa), and the mtDNA was also sequenced for one to eight individuals of the other sawfly species. The PCR reaction contained 2.5 μl of 10×Taq buffer, 2 μl of 25 mM MgCl2, 4 μl of 1.25 mM dNTPs, 12.25 μl of 1 mg ml−1 BSA, 1.25 μl of Taq Polymerase (Fermentas), 1.25 μl of 10 μM of primer HCO and LCO, 0.5 μl of DNA template to a total of 25 μl. Cycling conditions were: 95 °C for 5 min; 30 cycles at 95 °C for 45 s, 50 °C for 45 sec, 72 °C for 1 min; 72 °C for 10 min. PCR products were precipitated with 3M NaOAc and ethanol as described above for microsatellite development. Dried DNA pellets were commercially sequenced (Macrogen Inc.).
Analyses
Microsatellites were genotyped visually in Saga Generation 2 software (LI-COR). The number of alleles and genotypes, and expected heterozygosity were calculated in GENALEX 6 (Peakall & Smouse, Reference Peakall and Smouse2006). Mitochondrial DNA sequences were edited and aligned in Geneious Pro 5.3.4 (Biomatters Ltd, Auckland, New Zealand). Maximum likelihood phylogenetic trees were computed in MEGA version 5 (Tamura et al., Reference Tamura, Peterson, Peterson, Stecher, Nei and Kumar2011). The best model of molecular evolution was chosen using the maximum likelihood fits of different nucleotide substitution models. The substitution model with the lowest Bayesian information criterion (BIC) was the General Time Reversible model with gamma distributed rates and was used to compute a tree for the whole dataset with 100 bootstrap re-samplings. To assess if there was a relationship between percent divergence and the number of loci amplified, a linear regression was done with p-distance expressed as a percentage sequence difference between each haplotype and that of N. oligospilus from the invasive range, in SYSTAT 13 (Cranes Software International Ltd, Bangalore, India). To determine if microsatellite evolution had a directional bias and if smaller and larger alleles of heterozygotes were equally likely to mutate, Pearson's chi square tests for goodness-of-fit were used. A mutation was assumed to have occurred when a rare multilocus genotype differed at only one allele compared to a very common genotype (Wilson et al., Reference Wilson, Sunnucks and Hales2003).
Results
Microsatellite development
Of 87 clones sequenced, 79 (91%) contained microsatellite sequences. Six unclear sequences that contained microsatellites were discarded. Where clones yielded similar sequences, only one of each group was developed as a locus. Fifteen clones contained two microsatellite sections. AC repeats were by far the most common, with 61 clones containing between five and 23 repeats. GA, GAA or GAAAA repeats were also relatively common, with ten sequences ranging between four and 100 repeats. AAT and ATT were shorter and rarer; only six sequences contained them. Many of the microsatellite sections were impure (table 2). Four sequences containing minisatellites were also detected. All 43 loci could be successfully amplified using N. oligospilus DNA as PCR template. Two loci (WF1 and WF43) yielded undefined products and were discarded after initial screening. WF19 also gave inconsistent results and was eventually discarded.
Reproductive mode and genotypic diversity in N. oligospilus
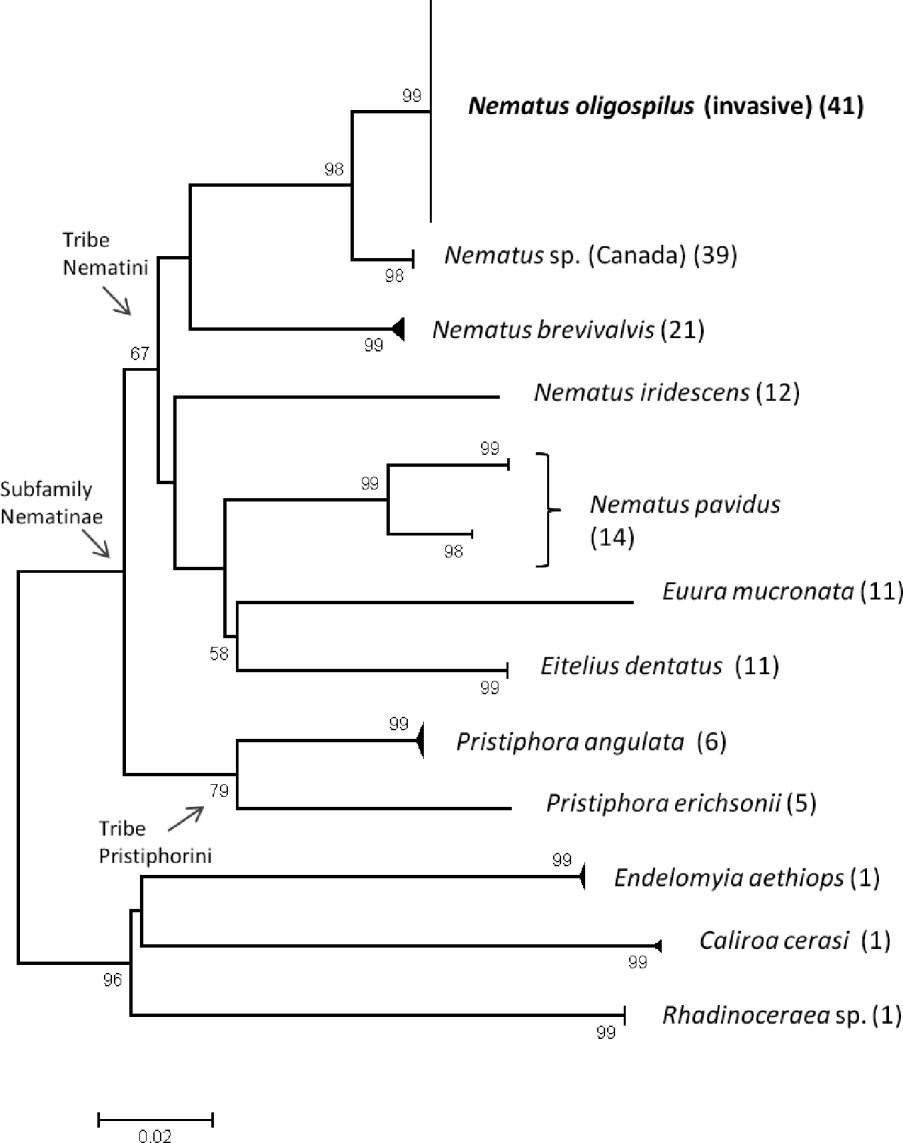
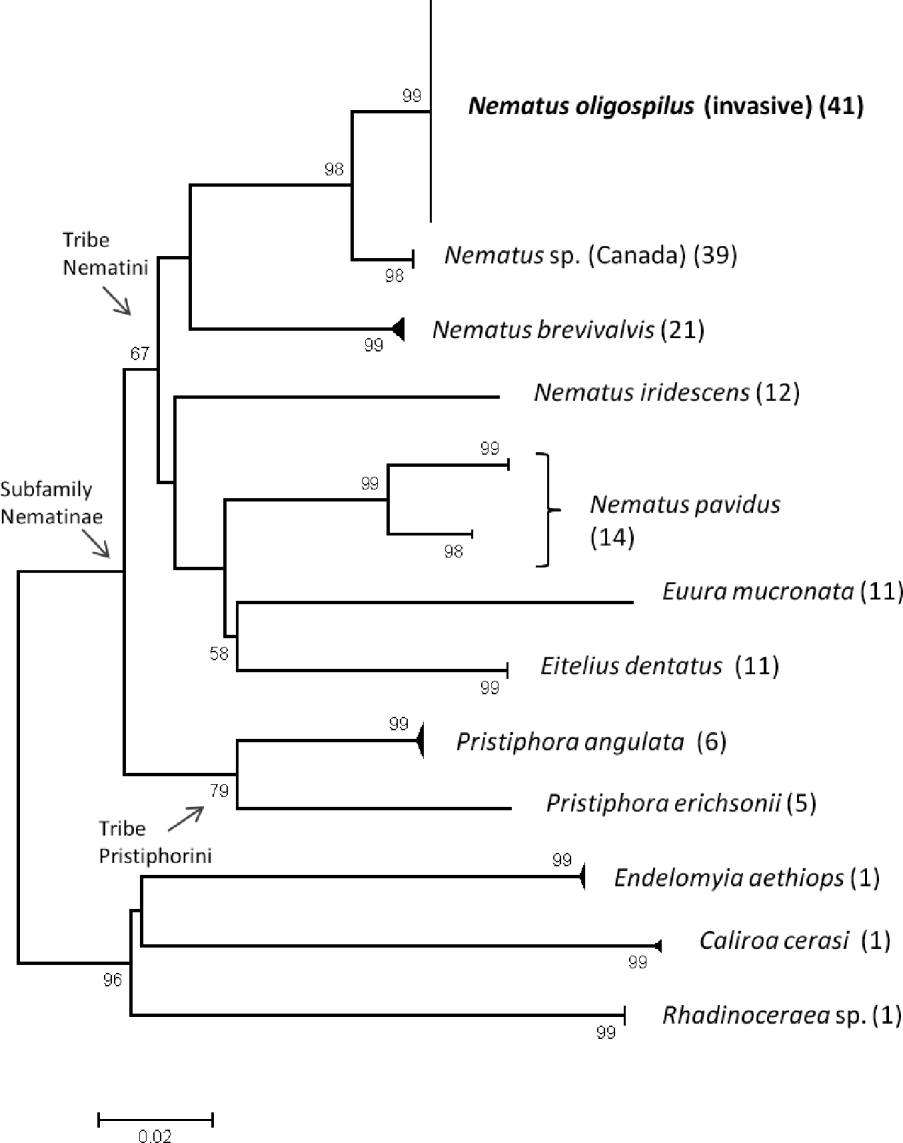
All N. oligospilus from the invasive range screened shared a single allele at 23 (56.1%) of the 41 loci tested. Of the remaining 18 loci showing heterozygosity, few alleles were found; for 14 loci, there were only two alleles, while WF2, WF4, WF35 and WF40 had three. Furthermore, a maximum of three genotypes per locus were identified in invaded range N. oligospilus (table 2). Of these, 18 heterozygous loci, seven presented the same heterozygote in all invaded range individuals, so 11 were useful to discriminate among genotypes of invasive range individuals. One main genotype was discerned from the invasive range. There were 16 other closely related genotypes, of which 14 were different from the common genotype at only one allele of one locus, while the other two genotypes were different at two loci. Differences between alleles were apparently due to single mutations with alleles losing or gaining one repeat. The mutational process did not have apparent directional size bias (Pearson χ2 = 1.0, df = 1, P = 0.317) and the smaller allele was not significantly more likely to undergo mutation than the larger allele (Pearson χ2 = 0.818, df = 1, P = 0.366). Low variation was also seen in mtDNA sequences; all N. oligospilus sequenced from South Africa, New Zealand and Australia had identical mtDNA sequences (fig. 1).
Maximum likelihood phylogeny of the sawfly species estimated applying the GTR-G substitution model for the mitochondrial DNA cytochrome-oxidase I sequences. The number of microsatellite loci amplifying for each species is given in parentheses.
Except for a single individual, all N. oligospilus in this study proved to be diploid (indicated by heterozygous loci) and are thus likely to be female. One apparent haploid individual (thus most likely a male) was detected during screening; the individual was collected as a larva, so could not be sexed physically. The lack of haploids combined with the distribution of a very common genotype and an array of rare, but closely related genotypes (despite considerable polymorphism) suggest that obligate or facultative parthenogenesis (‘functional parthenogenesis’) is by far the most likely reproductive mode for N. oligospilus in its invaded range. The low genotypic diversity is unlikely to be caused by low power in the genetic assay; the loci can readily distinguish different genotypes when they are present in other species (next section) and, with 18 multi-allelic loci, would detect new sexually-produced genotypes in the sampled invaded range with extremely high certainty.
Other sawfly species
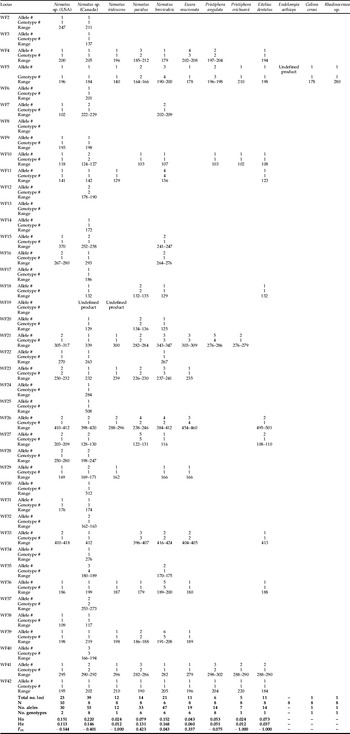
Many of the loci developed for N. oligospilus also amplified successfully in other sawfly species. Only two loci were specific to N. oligospilus. Most loci amplified in up to five of the species tested, and a few loci amplified in eight or more, including WF5 which amplified in all species tested (table 3). When they did amplify, most microsatellites had alleles unique to each species. Twenty-one loci revealed intraspecific variation, often in multiple species (table 3). Microsatellite loci useful in discriminating N. oligospilus genotypes were not more likely to differentiate between individuals of other species. Allele diversity was the highest for Nematus sp. (Canada) (53), followed by N. brevivalvis (47) and N. pavidus (33), despite low samples sizes (6–8), as compared with >1300 N. oligospilus. There was considerable genotypic diversity in these other species; most individuals bore different genotypes, with the exception of N. iridescens and Nematus sp. (Arizona, USA). This reinforces the low genotypic diversity of N. oligospilus, in which individuals nearly all had the same genotype (table 3). The majority of individuals of most sawfly species screened were heterozygous at some loci, indicating they were likely to be female and therefore would reproduce parthenogenetically. In two exceptions, N. brevivalvis and P. angulata, genotypic patterns were consistent with the presence of haploid males and diploid females.
Characteristics of microsatellite loci isolated from Nematus oligospilus screened on different sawfly species (number of alleles, number of genotypes, range of allele lengths). Empty cells indicate no amplification

The different sawfly species screened with the new microsatellite markers were related to N. oligospilus to different extents as estimated from mtDNA sequences (fig. 1). Members of the tribe Nematini formed a distinct group, while the tribe Pristiphorini formed a sister group. The three other species, Rhadinoceraea sp., C. cerasi and E. aethiops, were placed at the base of the tree in a less-defined cluster. The most closely related to N. oligospilus was Nematus sp. collected in Canada, while Nematus sp. collected in Arizona was in a sister clade with N. brevivalvis. Nematus pavidus COI sequences were monophyletic but fell in two distinct branches. Euura mucronata and Eitelius dentatus had modest support for grouping within Nematus.
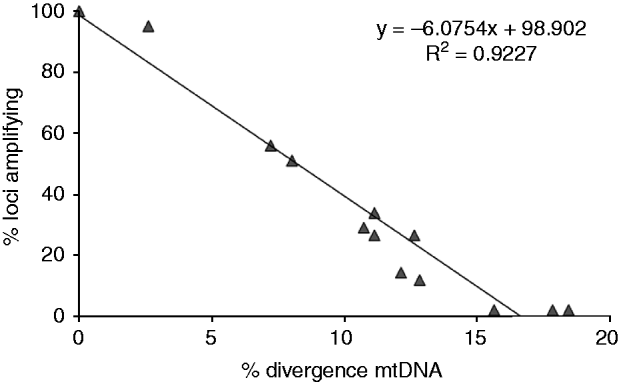
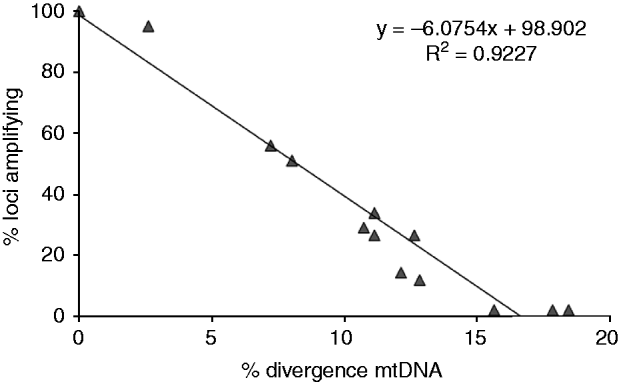
The percentage COI sequence divergence between invaded range N. oligospilus and other taxa was strongly negatively correlated with the percentage of loci amplifying in the other taxa (R2 = 0.92, F1,11 = 176.8, P < 0.001) (fig. 2). Successful amplification of loci in Nematus sp. varied between 29% for N. iridescens and 95% for the Nematus sp. from Canada, while Nematus sp. from Arizona, USA, had 56% success. The three more divergent species, Endelomyia aethiops, C. cerasi and Rhadinoceraea sp., each had only one locus amplifying (2.4%), while the success rate for Pristiphora species was ∼13%.
Relationship between the percentage of loci amplifying successfully and the percentage of interspecific sequence divergence as compared to the mitochondrial DNA cytochrome-oxidase I gene from Nematus oligospilus in the invasive range.
Discussion
Reproductive mode and clonal diversity in N. oligospilus
Some of the most successful invaders are parthenogenetic (e.g. Corrie et al., Reference Corrie, Crozier, Van Heeswijck and Hoffmann2002; Jokela et al., Reference Jokela, Lively, Dybdahl and Fox2003; Mergeay et al., Reference Mergeay, Verschuren and De Meester2006; Budde et al., Reference Budde, Gallo, Marchelli, Mosner, Liepelt, Ziegenhagen and Leyer2011). Nematus oligospilus is reported to be parthenogenetic in its invasive range (Urban & Eardley, Reference Urban and Eardley1995; Koch & Smith, Reference Koch and Smith2000), which is supported by the present data. Males are thought non-existent, but could be merely rare or morphologically unrecognized. The microsatellite markers suggest that N. oligospilus daughters are diploid and bear no recombined copies of their mother's microsatellite genotypes. Microsatellites indicated extremely rare haploid males in the invasive range – a single one was found in the >1300 individuals screened here. Although male(s) thus occur, their role is unknown; sexual reproduction has not been detected in this study according to the genotypic data. Given the number of variable loci, any new sexual recombination producing the screened individuals would have been detected very easily. Nematus oligospilus, therefore, can be recognized as a functionally parthenogenetic organism within its invasive range. Apomictic and automictic parthenogenesis can be hard to discern when using few molecular markers (Rabeling et al., Reference Rabeling, Lino-Neto, Cappellari, Dos-Santos, Mueller and Bacci2009), especially when recombination levels are very low (Kellner & Heinze, Reference Kellner and Heinze2011). In this study, the large number of microsatellite markers used showed no recombination, and heterozygosity was maintained; N. oligospilus is, therefore, unlikely to be automictic, and hence more likely to be apomictic (i.e. reproduces parthenogenetically by mitotic copying of the maternal genome). Parthenogenesis being the sole reproductive mode helps explain the fast population growth observed in previous studies in the Southern Hemisphere (Dapoto & Giganti, Reference Dapoto and Giganti1994; Urban & Eardley, Reference Urban and Eardley1995; Charles & Allan, Reference Charles and Allan2000; Ede et al., Reference Ede, Caron and Clements2007).
In its native range, N. oligospilus has sexual females and males (Koch & Smith, Reference Koch and Smith2000). Thus, the parthenogenesis experienced in the Southern Hemisphere is geographical, where parthenogenesis occurs only in some of the range of the organism. The native range of N. oligospilus is extensive, covering most of North America and Europe all the way to the Himalayas (Smith, Reference Smith, Krombein, Hurd, Smith and Burks1979; Liston, Reference Liston1995), and it is likely to represent a species complex (Schmidt & Smith, Reference Schmidt and Smith2009). We cannot discern if the species has a complete absence of sexual reproduction until native populations are assessed thoroughly. Two potential N. oligospilus populations were assessed in this study: Nematus sp. from Arizona and Montreal. When comparing mtDNA sequences, and considering the relatively modest proportion of microsatellite loci that amplified, Nematus sawflies collected in Arizona are likely to be a different species to N. oligospilus found in the Southern Hemisphere. The COI sequence divergence of 7.2% is in the range usually seen between members of different species of flying insects (e.g. Hebert et al., Reference Hebert, Cywinska, Ball and Dewaard2003, Reference Hebert, Penton, Burns, Janzen and Hallwachs2004; Park et al., Reference Park, Foottit, Maw and Hebert2011). In contrast, the Nematus sp. collected in Montreal had lower mtDNA sequence divergence (2.6%) and high microsatellite locus cross-amplification, and could be conspecific with N. oligospilus. Although, it is unknown if the source of N. oligospilus is parthenogenetic or if sexual reproduction occurs, the high genotypic diversity of Nematus sp. from Montreal indicates sexual reproduction in a close relative.
Genotypic (clonal) diversity is very low in the invasive range of N. oligospilus. The combination of microsatellites and mtDNA sequences in this study showed that the invasive sawfly found in South Africa, New Zealand and Australia are extremely genetically similar. They have apparently identical mtDNA sequences (certainly in the COI region), and microsatellite loci showed very similar (often identical as far as could be discerned) alleles and genotypes. Differences seen among N. oligospilus clones in the invasive range could be due to either the introduction of different clonal lineages or to mutations arising since introductions. Success of some invasive species has been attributed to the introductions of multiple clones, as in the pea aphid, Acyrthosiphon pisum Harris (Peccoud et al., Reference Peccoud, Figueroa, Silva, Ramirez, Mieuzet, Bonhomme, Stoeckel, Plantegenest and Simon2008). In the case of N. oligospilus, the low number of closely related clones and one widespread ‘main’ genotype suggest one or very few colonization events. In apomictic parthenogens, genotypes can be altered by mutations and chromosomal rearrangements (Loxdale, Reference Loxdale2010). Slippage mutation during the replication of DNA is the main mutational process occurring in microsatellites (Schlotterer & Tautz, Reference Schlotterer and Tautz1992). In N. oligospilus loci having more than one genotype, the difference between alleles of the main genotype and the novel alleles were the equivalent of losing or gaining a microsatellite repeat with equal probability. This shows that the differences in clonal lineages arose following non-directional mutations, at least roughly consistent with the stepwise mutation model, in which mutations are by single repeat slips rather than larger ones and unbiased in direction (Chambers & MacAvoy, Reference Chambers and MacAvoy2000). Further work is necessary to assess the spatial and temporal distributions of those clones, as well as their dispersal and host relationships.
Other sawfly species
Cross-amplification success of the new microsatellite markers was high for some other sawfly species tested. Relative to N. oligospilus, the proportions of additional genotypes discovered per individual screened were higher in some species, even though few individuals were screened for each species and most originated from a single site. Species such as C. cerasi are also thought to be parthenogenetic in Australia since males have not been collected (Naumann et al., Reference Naumann, Williams and Schmidt2002), while other species such as N. brevivalvis were inferred here to be sexual, showing more allelic diversity in a few individuals than N. oligospilus over a large part of its invasive range as here sampled.
As shown in other studies of broad taxonomic groups, here the more closely related to N. oligospilus a species was, the more successful microsatellite amplification (Zenger et al., Reference Zenger, Eldridge, Pope and Cooper2003; Primmer et al., Reference Primmer, Painter, Koskinen, Palo and Merilä2005). Overall, the genus Nematus and the tribe Nematini had high proportion of successful amplification. The Pristiphorini tribe had lower success, but most loci that did amplify revealed multiple alleles. A review on the success of cross-amplification of microsatellites shows that different taxonomic groups have different success rates. As a generalization for arthropods, over 60% of loci developed for a species will amplify in congenerics. This decreases rapidly for different genera in the same family (Barbarà et al., Reference Barbarà, Palma-Silva, Paggi, Bered, Fay and Lexer2007). Since largest genera in the Nematinae subfamily tend to be paraphyletic (Nyman et al., Reference Nyman, Zinovjev, Vikberg and Farrell2006b), it would not be judicious to predict the success of microsatellite markers at the level of genus; instead, the present results suggest that COI mtDNA sequence divergence is a very good predictor. In general though, microsatellite markers developed in this study are likely to be generally useful within the tribe Nematini, and still useful but less so for members of other tribes and subfamilies.
Due to their fairly high cross-amplification, carefully chosen microsatellite markers from the suite as here developed would allow the simultaneous study of several species, allowing comparison between species having different life strategies and reproductive modes (and indeed elucidating those modes in the first place). Furthermore, some genera such as Euura have been more thoroughly studied than others and already form strong model systems (Craig et al., Reference Craig, Price and Itami1992; Roininen et al., Reference Roininen, Price and Tahvanainen1996; Hjalten & Price, Reference Hjalten and Price1997; Nyman, Reference Nyman2002; McGeoch & Price, Reference McGeoch and Price2005; Price & Hunter, Reference Price and Hunter2005). Microsatellites used in conjunction with such models could be useful to test further ecological and evolutionary theories.
Conclusions
To manage an invasive species effectively, knowledge of its biology and ecology are essential. Reproductive mode and genotypic diversity can contribute to predicting impacts, distribution and population densities of invasive species. The present study showed that N. oligospilus is functionally parthenogenetic within its invasive range, with populations comprising only a small number of very closely related clones, which might go some way to explaining the rapid population growth seen in the introduced range (Caron, Reference Caron2011). In Australia and other Southern Hemisphere countries, N. oligospilus would appear to be an excellent study system for understanding evolution of invasive parthenogens that diverge without sexual reproduction. Furthermore, the microsatellites as developed represent useful tools for new and more highly-resolving approaches in well-established model systems, but also to study multiple species simultaneously.
Acknowledgements
We would like to thank colleagues for sharing samples (H. Roininen, C. Eardley, P. Price, C. Linnen and L. Kapari), A. Weeks for methodological advice, G. Perdomo, T. Hunt and D. Clements for technical assistance, A. Pavlova, C. Schmuki and T. Draper for useful discussions and H. Loxdale and an anonymous reviewer for helpful suggestions on the manuscript. This research was funded by Holsworth Endowment, the Department of Primary Industries Nancy Millis Postgraduate Award, North East Catchment Management Agency, West Gippsland Catchment Management Agency, North Central Catchment Management Agency and Melbourne Water.