Implications
Weaning (permanently or temporarily) shortly in advance of a ram exposure would improve the immediate ovulation response of lactating ewes in out-of-season breeding protocols.
Introduction
The success of accelerated lambing systems for prime lamb production is highly dependent upon rapid rebreeding of lactating or recently weaned ewes. Ewes in such systems are not expected to go through a dry period between weaning and the next mating period; they are rather expected to become pregnant before weaning, and as soon after parturition as manageable. Pharmacological protocols for inducing out-of-season reproduction in ewes are widely available. However, cost considerations, a discernible demand for environmentally friendly products, and an increasing awareness of ethical issues in reproductive control currently favour the application of more ‘natural’ means of assisting reproduction (Martin et al., Reference Martin, Milton, Davidson, Banchero Hunzicker, Lindsay and Blache2004; Martin and Kadokawa, Reference Martin and Kadokawa2006).
Exploiting the ‘ram effect’ has become the method of choice for overcoming seasonal anoestrus with nil or minimal pharmacological support. Rams, alone or in association with a small number of oestrous ewes, have proved effective at inducing ovulation during anoestrus in moderately seasonal breeds (Ungerfeld, Reference Ungerfeld2007). Lactating anovular ewes exhibited similar LH and ovulatory responses as did seasonally anovular ewes when exposed to rams under a favourable photoperiod (Poindron et al., Reference Poindron, Cognie, Gayerie, Orgeur, Oldham and Ravault1980), and the ram effect has been successfully applied for rebreeding autumn lambing ewes (Geytenbeek et al., Reference Geytenbeek, Oldham and Gray1984; Wright et al., Reference Wright, Geytenbeek, Clarke and Hoskinson1989).
Overcoming the simultaneous lactational and photoperiodic constraints experienced by ewes lambing in spring has proved more difficult. Rams, alone (e.g. Signoret et al., Reference Signoret, Fulkerson and Lindsay1982; Hamadeh et al., Reference Hamadeh, Abi-Said, Tami and Barbour2001) or associated with oestrous ewes (Silva and Ungerfeld, Reference Silva and Ungerfeld2006), have mostly produced modest results when spring rebreeding of lactating ewes has been attempted. Spring rebreeding necessarily occurs under adverse photoperiod so out-of-season reproductive strategies should focus on mitigating suckling effects, the main known inhibiting factor linked to post-partum anoestrus in ruminants (Williams, Reference Williams1990).
Suckling promotes the release of brain opioids (Malven, Reference Malven1986) that are partially responsible for the inhibitory effects of oestradiol upon the gonadotropin-releasing hormone-LH pathway (McNeilly, Reference McNeilly1994) thus maintaining the low LH pulse frequency typical of late gestation while delaying the resumption of cyclicity. Evidence for an effect of early permanent or temporary weaning on ovulation resumption in sheep is conflicting, with a few good (e.g. Restall, Reference Restall1971) and mostly poor (Signoret et al., Reference Signoret, Fulkerson and Lindsay1982; Hoefler and Hallford, Reference Hoefler and Hallford1987; Hamadeh et al., Reference Hamadeh, Abi-Said, Tami and Barbour2001) responses on record.
We report results from two exploratory studies, conducted with post-partum ewes of a moderately seasonal breed, aimed at assessing the potential of both permanent and temporary weaning for improving the ovulation and oestrus responses to the ram effect in spring. The main hypothesis underlying the studies was that the exclusion of lambs around the time of ram exposure would improve the response of post-partum anovular ewes.
Material and methods
Location, animals and general management
The experiments were conducted at the Argerich Experiment Station (latitude: 38° 44′S) using animals from an experimental Corriedale flock of approximately 350 dams. General management, experimental procedures and animal care were consistent with standards set in the Consortium guide (Consortium for Developing a Guide for the Care and Use of Agricultural Animals in Agricultural Research and Teaching, 1999). Ewes are regularly exposed to Corriedale rams every year from early to mid autumn (depending upon forage availability) with the bulk of lambing occurring from late August to late September. Shearing is pre-lambing and lambs are usually sold for the Christmas market straight from their dams in late December. Ewes graze native pastures year-round except during late gestation and early lactation when they graze winter crops (usually oats). During the course of the studies the ewes were kept isolated (sight, sound and smell) from adult males from the end of the mating period until the start of the experiments. Lambing was closely supervised in order to record date of lambing, number of lambs born to individual ewes, and lamb losses.
Two experiments were conducted in consecutive years involving the exposure of both recently weaned and matched (age, live weight, lambing date) post-partum non-lactating ewes (DRY) to the presence of rams and oestrous ewes. Mature ewes (n = 10) and vasectomised sexually experienced Corriedale rams wearing marking harnesses (10 in Experiment 1, 20 in Experiment 2) acted as the socio-sexual stimulus for the experimental animals. Ewes in these groups (different animals each year) were brought into standing oestrus when required by intramuscular injections of 500 μg of oestradiol propionate after a 7-day progestagen priming period (intravaginal sponges impregnated with 40 mg of medroxyprogesterone acetate) and introduced to the experimental animals early in the morning (Martin et al., Reference Martin, Cognié, Schirar, Nunes Ribeiro, Fabre-Nys and Thiéry1985). Ten additional oestrous ewes were added to the stimulus group after the first 24 h of exposure.
Design and experimental procedures
Experiment 1
Figure 1 shows the timing of main experimental interventions in both studies. In Experiment 1, 130 lactating ewes (evidence of current suckling at udder examination confirming a survival record for a single-born lamb, or for at least one lamb in multiple litters) were randomly assigned to four experimental units on the basis of age (2 to 7-year-old ewes), live weight (54 ± 6.9 kg; mean ± s.d.), and date of lambing (September 16 to October 18). These units were then randomly allocated to four weaning treatments: dams separated from their lambs immediately before being exposed to the stimulus group on day 0 (W-0), or 1 (W-1), 2 (W-2), or 4 (W-4) days before that. Another 75 non-lactating flockmates (evidence of udder involution and no recent suckling confirming a record of lamb loss after parturition) were screened (same variables used for the stratification of the lactating group) to produce a matching group of DRY ewes (n = 32). In order to minimise discomfort, animal suffering, and chances of mismothering, anovulation of experimental ewes was not verified before ram exposure. It would be unlikely for a post-partum Corriedale ewe to spontaneously ovulate in the middle of the seasonal anoestrus, and absence of any recent ovulation activity was confirmed retrospectively at first laparoscopy after ram exposure. Experimental ewes were exposed to the stimulus group in a 0.3 ha enclosure for 5 days and then in a 20 ha paddock for another 23 days.
Time line of dates and time elapsed relative to ram introduction detailing experimental events and recording of end-point variables for Experiments 1 and 2. ‘Lap’ stands for exploratory laparoscopy.

The occurrence of oestrus in experimental ewes (as assessed by rump marks) was recorded daily until day 5, every 3 to 4 days until day 17, and daily again from day 17 to day 28. Mid-ventral laparoscopy, performed under local anaesthesia after an overnight fasting, was used to determine occurrence and timing of ovulation (on the basis of colour of the corpora lutea present on the surface of the ovaries; Oldham and Lindsay, Reference Oldham and Lindsay1980) on day 5 in all ewes exposed, and on day 28 in all ewes not showing oestrus during the experimental period (i.e. including those not responding with ovulation as assessed on day 5).
Experiment 2
As in Experiment 1, lactating (n = 230) and matched post-partum DRY ewes (n = 54) were used. Lactating ewes were randomized by strata to eight experimental units according to age (2 to 7-year-old ewes), live weight (50 ± 5.3 kg; mean ± s.d.), body condition score (2.3 ± 0.37, mean ± s.d.; scale 1 (emaciated) to 5 (obese); Jeffries, Reference Jeffries1961), and date of lambing (August 5 to September 10). Units were then randomly allocated to an unreplicated two-factor factorial arrangement consisting of two levels of temporary weaning applied before the start of the exposure period (B0: control, no temporary weaning; B24: ewes have their lambs removed 24 h before stimulation) and four levels of ewe-lamb contact at the start of stimulation (A0: control, ewes exposed to rams while in contact with their lambs; A12, A24 and A36: ewes not in contact with their lambs for the 12, 24 or 36 initial hours of ram exposure).
Imposing treatment combinations demanded splitting and rejoining groups of dams and lambs from 24 h before to 36 h after the start of the stimulation. Young lambs are notoriously difficult to manage so, in order to minimise stress and chances of unwanted mother-lamb separations, two contiguous enclosures separated by a wire fence were used to manage the animals while imposing the treatments. All lambs were initially kept as a single mob in one of the enclosures, in the company of part of the experimental ewes (starting with DRY and B0 ewes 24 h before the ram exposure); their dams were then moved in according to protocol, from the other enclosure. Seven lambs managed to join their dams ahead of schedule; those ewes were maintained with the experimental groups but discarded for analyses.
The socio-sexual stimulus group of 20 rams and 10 oestrous ewes (10 additional oestrous ewes added 24 h later) was initially split proportionately to ewe numbers in the enclosures and joined in early morning on day 0. Proportions were then adjusted every 12 h by moving rams and oestrous ewes along with the experimental ewes scheduled to rejoin their lambs at every set time. Ovulation and oestrus were monitored as described for Experiment 1, except that oestrus was recorded from days 16 to 28 and the second laparoscopy was performed on day 32 on a 50% sample of ewes not marked by the rams after an initial ovulation response (as assessed on day 5).
Statistical analyses
The χ 2 or Fisher’s exact tests (when the expected count for any cell was < 5) were used for comparing proportions; ovulation rates were compared using Brown (Reference Brown1988) procedure. Four pre-planned comparisons were performed in Experiment 1: dry (DRY) v. recently weaned (W-4, W-2, W-1 and W-0) ewes, an overall comparison among recently weaned ewes (W-4, W-2, W-1 and W-0), weaned before (W-4, W-2 and W-1) v. weaned on the day of socio-sexual exposure (W-0), and another overall comparison among groups weaned before socio-sexual exposure (W-4, W-2 and W-1). Means and proportions for lactating and DRY ewes in Experiment 2 were compared using the same procedures. The unreplicated factorial array of lactating ewes (i.e. B and A factors excluding the DRY group) was then subjected to two-way ANOVA by fitting B and A effects plus a 1-d.f. factor testing for lack of additivity (Tukey, Reference Tukey1949); diagnostic plots were also applied to explore for a possible lack of additivity of B and A effects. Confidence intervals (0.05 family-wise error rate) were calculated for the differences between levels of lamb-ewe contact as the start of stimulation (A12, A24 and A36) against their control (A0) using the Bonferroni method.
As a consequence of the time arrangement of the B and A factors, the total time lambs were separated from their dams varied from 0 (B0–A0 combination) to 60 h (B24–A36 combination) with two replicated combinations (i.e. 24 h for B0–A24 and B24–A0; 36 h for B24–A12 and B0–A36) in between those extremes. Possible effects of this factor (total time dams were separated from their lambs) on the variables recorded were explored: (i) by regressing (linear and quadratic terms) response variables against the time mothers were not in contact with their lambs and (ii) by including the factor as a covariate in the linear model when testing for B and A effects. The same procedure was applied for post hoc assessment of possible effects of timing of lamb restitution relative to the day-night cycle.
Logistic analysis (McCullagh and Nelder, Reference McCullagh and Nelder1989) of response variables regressed against date of lambing was also applied for post hoc exploration of potential trends associated to time since lambing in both experiments. S-Plus 2000 (MathSoft Inc., 2000) was used for calculations.
Results
Experiment 1
No indication of cyclic activity previous to the exposure to rams and oestrous ewes (i.e. corpora albicantia or corpora lutea older than 3 to 4 days present on the surface of the ovaries) was detected for any ewe at laparoscopy on day 5. Ovulation and oestrous responses of DRY and recently weaned ewes were similar for all variables analysed (Table 1). The immediate ovulation response to the socio-sexual stimulus tended to be lower (P = 0.065) in ewes weaned on day 0 (71.9%) than among the rest of recently weaned ewes (87.8%, 86/98) but this occurred in the context of a non-significant overall test among weaned ewes (P = 0.18; Table 1). Differences in ovulation rate among recently weaned ewes (P = 0.003), among ewes weaned before day 0 (P = 0.044), and between W-0 and the rest of recently weaned ewes (P = 0.006) were traced to the comparatively low mean ovulation rate recorded in W-2 ewes (Table 1).
Experiment 1. Reproductive responses of recently weaned Corriedale ewes (W) and matching dry flockmates (DRY) exposed to rams and oestrous ewes in late spring

W-0, W-1, W-2, W-4 = ewes weaned 0, 1, 2, or 4 days before ram exposure on December 6; DRY = matching group of post-partum non-lactating ewes.
aOne ewe removed for health reasons in W-0, one ewe in W-1 and two in W-4 were not present at laparoscopy.
No ewes other than those in the stimulus group were detected in oestrus before day 17. The occurrence of induced oestrus was similar among weaned ewes (Table 1); pre-planned comparisons for this variable were all far from significant. The distribution of marked ewes was bimodal (data not shown) with a strong bias towards late rather than early oestrus occurrence over the control period; 29.7% (22/74) of marked ewes were detected from day 17 to day 21 v. 70.3% (52/74) between days 22 and 26 (P < 0.02). This trend was similar (P = 0.83) for both DRY and lactating ewes.
None of the 24 initially unresponsive ewes (i.e. anovular on day 5) showed oestrus during the control period or exhibited any sign of ovulation activity on day 28. Irrespective of weaning treatment, similar (P = 0.24) proportions of ewes had reverted to anovulation by day 28. Relative to the initial number of ewes exposed, more ewes (P = 0.011) were still cycling by day 28 (i.e. marked ewes plus ewes having recently formed corpora lutea at laparoscopy on day 28) when weaning occurred one or more days before (80%, 76/95) rather than at ram exposure (54.8%).
Experiment 2
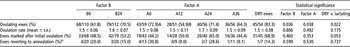
One lactating ewe having a recently formed corpus albicans at laparoscopy on day 5 was removed from the experiment; no other indication of ovulation activity previous to the introduction of rams was detected. DRY ewes showed higher (P = 0.022) immediate ovulation response (83.3%) and expression of oestrus (68.9%, P < 0.053) than lactating ewes (66.2% (147/222) and 51% (75/147), respectively); ovulation rate (1.5 ± 0.05 v. 1.5 ± 0.08) and the proportion of ewes reverting to anovulation by day 32 (14.3% v. 17.5% (7/40)) were similar (P = 0.175 and P = 0.737, respectively) between those groups (Table 2).
Experiment 2. Reproductive responses of lactating Corriedale ewes and matching dry flockmates (DRY) exposed to rams and oestrous ewes in mid spring

B0, B24 = control, lambs removed 24 h before stimulation; A0, A12 to A36 = control, ewes not in contact with their lambs for the 12 to 36 initial hours of ram exposure; DRY = matching group of post-partum non-lactating ewes.
aDetermined on a 50% sample of non-marked ewes.
A, B: different letters are significantly different (P < 0.05).
Differences within the temporary weaning factorial array were only detected for immediate ovulation following ram exposure (Table 2) and there was no indication of lack of additivity for the effects of the B and A factors on this or any other variable (P > 0.25, Tukey’s 1-d.f. test). More ewes ovulated within 5 days when lambs were separated from their dams for 24 h before ram exposure; this effect was modest (B24: 70.5 v. B0: 61.8, Table 2) but consistent across levels of the A factor and, hence, significant (P = 0.036). Differences were also detected associated to the time lambs were not allowed to get in contact with their dams during the initial hours of ram exposure (P = 0.038, Table 2). Comparisons against the control level for the factor (A0, 72.9%) showed a lower ovulation response (95% CI for the difference excluding 0) in ewes having their lambs returned 12 h after the onset of the ram exposure (A12, 54.9%); no other comparisons differed.
When total time of lamb-ewe separation (0 to 60 h depending upon B–A level combinations) was fitted as a covariate in the linear model describing ovulation (only variable affected by the experimental factors) it was found not significant (P = 0.16), and the significance of the B and A factors themselves was barely modified. The time lambs spent away from their dams explained < 11% of total variation for any of the other response variables and none of the estimated regression coefficient was different from 0. In contrast, fitting a two-level factor representing the day-night cycle (morning for A0 and A24, evening for A12 and A36) explained (P < 0.04) a significant portion (53%) of the variation recorded in ovulation response. This effect was independent of the B factor (no change in statistical significance) but turned the A factor into a non-significant (P = 0.46) source of variation when fitted together in a linear model.
As found in Experiment 1, the oestrous distribution was biased towards late occurrence (P < 0.03) with fewer ewes marked by the rams before (36/106; 34.0%) rather than after (70/106; 66.0%) day 22. The trend did not differ (P = 0.66) between DRY and lactating ewes.
For both experiments, logistic regression analyses did not detect any association (P > 0.3) between the extension of the post-partum period for individual ewes and the response variables evaluated in the studies.
Discussion
The first experiment investigated ovulation and oestrous responses of recently weaned ewes and a matched group of post-partum flockmates that, having lambed over the same period, subsequently lost their lambs. These two groups are relevant for reproductive management as both, lactating and naturally occurring dry post-partum ewes, are required to rebreed during seasonal anoestrus in accelerated lambing systems. Building upon results from Experiment 1, the second trial explored variations of a critical aspect of temporary weaning: when to keep ewes separated from their lambs. The rationale for the second experiment was (i) to better quantify the effect of removing lambs from lactating ewes before ram exposure and (ii) to assess the consequences of temporarily maintaining ewes away from their lambs while exposing them to a stimulus group of rams and oestrous ewes. We hypothesised that excluding the lambs during the critical period of increased LH frequency typical of a sudden exposure of Corriedale ewes to rams (Ferrería et al., Reference Ferrería, Rodríguez Iglesias, Pevsner, Aba, Rodríguez and Pedrueza2008) could mitigate the adverse effects associated to suckling.
In both experiments, the proportion of DRY ewes showing an immediate ovulation response after 5 days of contact with the stimulus group was comparable, though somewhat lower, to what has been reported for non-lactating, seasonally anovular Corriedale ewes (90% to 95%, Rodríguez Iglesias et al., Reference Rodríguez Iglesias, Ciccioli and Irazoqui1991, Reference Rodríguez Iglesias, Ciccioli, Irazoqui and Ciccioli1996 and Reference Rodríguez Iglesias, Ciccioli, Irazoqui and Rodríguez1997). However, a sizeable proportion of initially ovulating DRY ewes was not marked by the rams during the control periods (45% in Experiment 1, 31% in Experiment 2), which is in contrast to the usually high proportion of Corriedale ewes marked after a successful stimulation during seasonal anoestrus (e.g. Rodríguez Iglesias et al., Reference Rodríguez Iglesias, Ciccioli and Irazoqui1997). Although comparisons between experiments may be confounded by other factors, the magnitude and consistency of the differences, and the low proportion of DRY ewes reverting to anovulation amongst those not marked by the rams (1/13 in Experiment 1 and 1/7 in Experiment 2), suggest that a recent history of pregnancy and lamb raising may probably affect the expression of behavioural oestrus after a successful ovulation response.
DRY and recently weaned ewes in Experiment 1 showed similar immediate ovulation responses (90.6% v. 83.9%, respectively). This contrasts with the marked difference observed between DRY (83.3%) and lactating (66.2%) ewes in Experiment 2. We hypothesise that the presence of the lambs may explain those differences. Suckling has been suggested to delay the onset of cyclicity after parturition (Mauléon and Dauzier, Reference Mauléon and Dauzier1965; Restall, Reference Restall1971; Shevah et al., Reference Shevah, Black, Carr and Land1974) by promoting the release of brain opioids (Malven, Reference Malven1986) which, in turn, affect LH secretion via the inhibitory effect of oestradiol (McNeilly, Reference McNeilly1994). Removing the suckling stimulus in Experiment 1 may have facilitated the rapid increase in LH frequency required for a ram-induced ovulation to occur (Poindron et al., Reference Poindron, Cognie, Gayerie, Orgeur, Oldham and Ravault1980). The overall significance of the effect of the time ewes spent away from their lambs while exposed to rams in Experiment 2 also points towards lamb interference, possibly through suckling, acting upon LH pulsatility. LH pulse frequency increases dramatically upon ram exposure (Poindron et al., Reference Poindron, Cognie, Gayerie, Orgeur, Oldham and Ravault1980) and sustained pulsatility is critical for a ram-induced preovulatory LH surge to occur, usually within 24 to 36 h (Martin et al., Reference Martin, Oldham, Cognié and Pearce1986). The logistics of Experiment 2 precluded any attempts of monitoring suckling patterns across experimental groups, which could have helped at explaining the depressed ovulation response recorded in A12 ewes. However, it is difficult to reconcile the pattern of ovulation responses recorded across levels of factor A with some altered suckling behaviour only affecting lambs reunited with their dams precisely 12 h after the start of the stimulation. The existence of a critical temporal window for LH secretion interference is another possibility; ewes in A12 may have been traversing such a window when their lambs were returned to them around 12 h into the period of ram exposure. However, ewes in A0, also in contact with their lambs around 12 h after the start of the stimulation, did not experience any depression of their ovulation response. Thus, in order to fit the observed pattern of ovulation responses across groups, the hypothesis of a critical temporal window should be complemented with some interacting effect of, for example, higher suckling intensity in A12 than in A0, possibly due to the recency of lamb restitution in A12. That would make the critical window hypothesis less likely although it might probably deserve further investigation.
The lower ovulation response observed among A12 ewes could have also been induced by the timing of lamb restitution relative to the day-night cycle (i.e. after sunset) for that particular group. Returning lambs during the night may have been particularly stressing for the ewes; the process of pair bonding may have taken longer (e.g. due to limited vision), and interference with the normal circadian rhythm of activity may have also contributed to impair the critical LH secretion pattern. The other experimental group to which lambs were returned at night (A36) also showed a somewhat lower ovulation response (64.3%) than the groups that had their lambs returned during the morning hours (72.9% and 71.4%, respectively, for A0 and A24); this is consistent with the hypothesis of a possible daytime effect. On the other hand, any effect of timing of lamb restitution in A36 would be expected to be less noticeable than in A12 because many A36 ewes might have already experienced their LH surges by the time (Martin et al., Reference Martin, Oldham, Cognié and Pearce1986) lambs were returned to them. The post hoc analysis performed by testing the significance of a two-level factor representing the day-night cycle supports timing of lamb restitution relative to the day-night cycle as a likely cause of the depressed ovulation response of A12 ewes. Further research will be required to determine ultimate causes and possible pathways of lamb interference in the endocrine response of lactating ewes to the presence of rams.
Mean ovulation rates in both experiments were comparable to peak breeding season values for the breed (e.g. Rodríguez Iglesias et al., Reference Rodríguez Iglesias, Irazoqui, Ciccioli and Giglioli1993), a common finding for ram-induced ovulation of non-lactating seasonally anovular ewes (Martin et al., Reference Martin, Oldham, Cognié and Pearce1986). Differences in ovulation rate detected in Experiment 1 were mainly associated with the comparatively low figure recorded for W-2 ewes. Although a biological explanation for such a difference should not be dismissed, we failed at finding a likely cause for the lower figure observed only in ewes weaned precisely 48 h before exposure. The absence of any discernible temporal pattern in group-wise unreplicated Experiment 1, compared to the homogenous ovulation rate response observed in (group-wise replicated) Experiment 2, suggest that sampling error may has been involved in the resulting observed difference.
Effects of a pre-exposure weaning on the ovulation and oestrous responses to the introduction of rams (W-0 v. recently weaned ewes in Experiment 1; B0 v. B24 ewes in Experiment 2) have not been reported before. Our results suggest a modest but consistently beneficial effect of weaning the lambs, either temporarily or permanently, before exposing their dams to the rams. Removing the lambs before ram exposure increased the immediate ovulation response (both experiments), and the proportion of ewes still cycling by day 28 (Experiment 1). Advancing lamb removal for 2 or 4 days before ram exposure did not accrue any significant additional improvement in the response variables (Experiment 1). This suggests that the effect of pre-exposure weaning is also probably due to the exclusion of suckling as an inhibiting factor acting upon LH secretion. The difference detected in the proportion of ewes marked between DRY (68.9%) and lactating (51.0%) ewes in Experiment 2, and the fairly similar oestrous occurrence in both DRY and recently weaned ewes in Experiment 1 (55.2% and 53.7%, respectively) also supports the notion of lamb suckling interfering with both ovulation and oestrous behaviour. Thus, characterising both ewe-lamb behaviour during the period of initial ram exposure (i.e. first 24 to 36 h) and ewe-lamb-ram interactions around the expected period of first induced oestrus, seem to be critical experimental goals for understanding the constraints involved in ram-induced reproduction of lactating ewes. Lamb interference on mating behaviour (possibly effected through an induced decline of ewe proceptive behaviour) could be minimised by combining low-dose short-term exposure to progesterone (Rodríguez Iglesias et al., Reference Rodríguez Iglesias, Ciccioli and Irazoqui1997), applied in advance to ram exposure, and temporary lamb removal around the expected time of first induced oestrus and ovulation. Such a protocol would also capitalise on the relatively higher ovulation rate expected at the first induced ovulation. The lack of any further improvement of reproductive variables from advancing lamb removal for 2 or 4 days before ram exposure also supports the concept of temporary weaning coupled with low-dose short-term progesterone priming as the protocol of choice for ram inducing lactating ewes.
We did not detect any significant association between variation in post-partum interval of individual ewes and ovulation and oestrous responses to the ram effect. That leaves lamb suckling behaviour as the key factor controlling responsiveness of lactating ewes to the ram effect. However, other variables affecting both lactating and dry post-partum ewes are probably involved in the relatively poor oestrous responses recorded in both experiments. Oestrus distributions biased towards late rather than early occurrence in both experiments are indicative of a high incidence of corpora lutea with a short life span (Oldham and Lindsay, Reference Oldham and Lindsay1980), a type of response associated to deep anoestrus (Chemineau et al., Reference Chemineau, Pellicer-Rubio, Lassoued, Khaldi and Monniaux2006) probably induced, in this case, by the simultaneous operation of both post-partum and photoperiodic constraints.
Conclusions
(i) The poor response of lactating ewes to the introduction of rams in spring is confirmed; (ii) suckling seems to be a key depressing factor of both ovulation and oestrous responses, which warrants extensive research of ewe-lamb behaviour during initial ram exposure, and of ewe-lamb-ram interactions around oestrus; (iii) separating mothers from lambs for at least 24 h before ram exposure will probably improve the chances of inducing ovulation; (iv) until further information on hormonal and behavioural interactions becomes available, lamb restitution during night hours should be avoided in protocols of temporary weaning.
Acknowledgements
This study was partially supported by grant PICT 08-12411 from ANPCyT, Argentina. Technical assistance from Héctor Larrea, Jorge Kellerer, Carlos Colitripai, Nick B. Collie and María Manuela Rodríguez is gratefully acknowledged.