Introduction
Fishes display a wide range of reproductive strategies that are influenced by environment and seasonal changes influencing the physicochemical properties of the water. Oviparity is the most common mode, in which females release eggs into the water that are subsequently fertilized by males (Mokhtar, Reference Mokhtar2025). To maximize offspring survival, many species employ an R-selection strategy, producing a large number of eggs with minimal or no parental care (Pianka, Reference Pianka1970; Reznick et al., Reference Reznick, Bryant and Bashey2002). In contrast, species with a K-strategy produce fewer by larger eggs, typically deposited in protected sites and frequently accompanied by some degree of parental care (Pianka, Reference Pianka1970; Reznick et al., Reference Reznick, Bryant and Bashey2002).
They also exhibit developmental plasticity in the timing of embryogenesis and hatching, which functions as an adaptive mechanism enhancing offspring survival in unpredictable environments, particularly in temporary or highly variable aquatic systems (Mignien and Stoll, Reference Mignien and Stoll2024). One such strategy is diapause, a state of arrested development that can occur at specific stages of embryogenesis, allowing embryos to survive prolonged periods of unfavorable conditions until environmental cues trigger the resumption of development (Wourms, Reference Wourms1972). In contrast, retarded hatching occurs when embryos are fully developed but remain inside the chorion until external factors, such as hydrological or physicochemical changes, stimulate emergence (Wourms, Reference Wourms1972; Thépot and Jerry, Reference Thépot and Jerry2015).
Within Siluriformes, the family Loricariidae stands out as the most species-rich group, comprising 1069 valid species (Fricke et al., Reference Fricke, Eschmeyer and Fong2025) that are currently arranged into six subfamilies: Lithogeninae, Delturinae, Rhinelepinae, Loricariinae, Hypoptopomatinae, and Hypostominae (Lujan et al., Reference Lujan, German and Winemiller2015; Silva and Rapp Py–Daniel, Reference Silva and Rapp Py–Daniel2018; Roxo et al., Reference Roxo, Ochoa, Silva, Lujan, Tagliacollo, Britzke, Melo, Foresti, Oliveira and Albert2019; Londoño-Burbano and Reis, Reference Londoño-Burbano and Reis2021; Van der Laan et al., Reference Van der Laan, Fricke and Eschmeyer2026). Members of this family occupy a wide range of freshwater habitats throughout South America and the southern portion of Central America (Armbruster, Reference Armbruster2004; Weber et al., Reference Weber, Covain and Fisch-Muller2012; Lujan et al., Reference Lujan, German and Winemiller2015).
The phenotypic diversity of Loricariids represents one of the largest groups of freshwater ornamental fish available in the market. Consequently, the trade is predominantly reliant on wild-caught individuals, which do not fully represent the diversity found within these groups (Novák et al., Reference Novák, Hohl, Stuchlík, Hofmann, Tlusty, Magalhães, Maceda-Veiga, Akmal, Yue, Kumkar, Marr, Sara, Stern, Rhyne, Furse, Kalous and Patoka2025; Sassi et al., Reference Sassi, Cioffi and Moreira-Filho2025). However, breeding these species in captivity remains a significant challenge. Their K-strategy reproductive behavior is closely linked to environmental factors and water characteristics during the breeding season. Loricariids spawn in specific microhabitats, where eggs are deposited and guarded by males that provide parental care within caves or nests. The large, yolk-rich eggs remain protected until larval development is complete (Pianka, Reference Pianka1970; Mignien and Stoll, Reference Mignien and Stoll2024; Viana et al., Reference Viana, Abe, Oliveira, Rocha, Reis and Servili2025).
The Atabapo butterfly pleco Dekeyseria picta (Kner, Reference Kner1854) is a loricariid of commercial importance in the ornamental fish trade. This species inhabits blackwater environments associated with fast-flowing habitats, commonly found among submerged wood or rocky substrates in the Negro and Orinoco basins (Silva and Rapp Py–Daniel, Reference Silva and Rapp Py–Daniel2018). Knowledge of its reproductive biology remains limited; however, reproductive males show hypertrophied odontodes on cheeks, body, and fins. Furthermore, males exhibit parental care, covering the clutch during reproduction with their enlarged pelvic fins (Silva and Rapp Py–Daniel, Reference Silva and Rapp Py–Daniel2018).
As an important ornamental species, Dekeyseria picta is a focal species of the REDD + Matavén project, a United Nations initiative aimed at mitigating climate change through the reduction of CO₂ emissions from deforestation while promoting biodiversity conservation and sustainable livelihoods. In collaboration with the Foundation FUNINDES Colombia (Fundación para la Investigación y el Desarrollo Sostenible), this study was conducted to reproduce D. picta under captive conditions, addressing the lack of reproductive information for this species and contributing to the preservation of a resource threatened by overfishing and climate change.
Aquaculture and controlled reproduction provide essential baseline biological data for understudied Neotropical fishes of ornamental and conservation interest (Novák et al., Reference Novák, Hofmann, Hohl, Magalhães and Patoka2022). The documentation of reproductive traits and early embryonic development offers valuable insights into developmental plasticity and reproductive strategies (Bertolini et al., Reference Bertolini, Lopez, Nascimento, Arashiro, Silva, Santos, Senhorini and Yasui2020). In this context, the present study reports the first successful captive breeding of D. picta and describes its embryonic development as a foundation for conservation, sustainable ornamental fisheries, and future aquaculture-based management efforts.
Material and methods
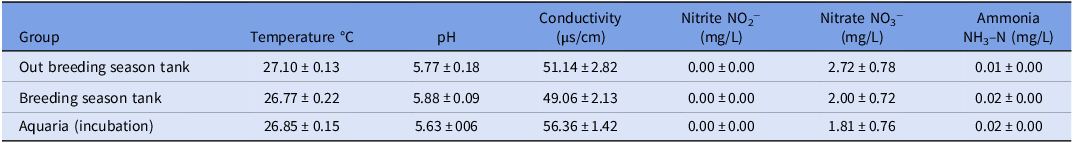
Specimens were obtained from the wild through indigenous fishers in the Matavén stream (4°31′44.7″ N, 67°52′07.4″ W) in June 2023. Ten females and nine males (9.74 ± 0.06 cm) were captured by freediving using a mask and flashlight and subsequently transferred to captivity. After capture, fish were transported to the Centro de Desarrollo Tecnológico de Peces Ornamentales de la Selva del Matavén (CDTPM) in Inírida – Guainía, Colombia, and acclimated together in a single 1000-L tank operated under a recirculating aquaculture system (RAS) equipped with a canister filter (EF-1200U, Resun®, China) and artificial clay caves measuring approximately 13 cm in length and 7 cm in width. During acclimation and throughout the experimental period, water temperature was monitored and maintained as reported in Table 1, and a controlled photoperiod of 12 h light and 12 h darkness was applied. Broodstock were fed once daily in the evening with a commercial sinking pellet (Omega One® Super Color Sinking Pellets,), containing 39.4% crude protein, 13.37% crude fat, 1.68% crude fiber, 1.82% omega-3, and 1.18% omega-6.
Water parameters measured prior to and during breeding season of Dekeyseria picta

Water parameters were monitored daily, including conductivity, measured with a handheld device (Health Metric TDS-EC, Health Metric®, USA), and temperature and pH, recorded using a pH tester (HALO 2, Hanna Instruments®, Romania). Ammonia was measured weekly using an ammonia checker (HI700 Ammonia Low Range, Hanna Instruments®), total hardness with test strips (Sofcheck, Hach®, USA), and nitrite (NO₂⁻) and nitrate (NO₃⁻) with a colorimetric test kit (API Fish Care®, USA). Approximately 50% of the water in the broodstock tank was replaced weekly to compensate for evaporation and to remove fish waste.
The animals were maintained under these conditions for eight months, until the rainy season began. Spawning events then occurred at a male-to-female ratio of 9:10, without the use of external hormonal induction. Eggs were collected by carefully detaching them with a spatula or by siphoning when they became loose at the tank bottom. At the time eggs were introduced, the 30-L incubation aquaria were filled with water from the broodstock tank to ensure identical environmental conditions. Continuous aeration was provided using a porous air stone. Partial daily water exchanges (20%) were performed. Water temperature, pH, conductivity, and nitrogenous compounds (ammonia, nitrite, and nitrate) during incubation are reported in Table 1. Each spawn was incubated separately to ensure precise data collection.
For monitoring embryo development, a sample consisting of three eggs from each spawning was observed in a stereomicroscope (STEMI DV4, ZEISS®, Germany) and photographed with an external camera. The measurements were evaluated using ImageJ® software v.1.51p.
Statistical analyses were applied exclusively to water quality parameters. Normality and homoscedasticity were assessed using the Kolmogorov–Smirnov–Lilliefors and Levene tests, respectively. When assumptions were met, comparisons among sampling periods were performed using one-way ANOVA; otherwise, the Kruskal–Wallis test was applied. The significance level was set at p < 0.05. All analyses were conducted using GraphPad Prism 5.0 (GraphPad Software, San Diego, CA, USA). Biological observations related to egg morphology, egg size, and embryonic developmental stages were analyzed descriptively. Results are presented as mean ± standard error of the mean (SEM).
Results
A total of 21 spawning events were analyzed between February and May of 2024, coinciding with the rainy season. The exact timing of spawning could not be determined, as oviposition occurred predominantly during nighttime or early morning hours. To avoid disturbing wild-caught broodstock during their first successful reproduction in captivity, spawning caves were inspected once daily in the morning. Water parameters did not differ significantly (Table 1); however, during breeding activity, reductions in temperature and conductivity, together with increases in pH, were observed.
The eggs were spherical and featured a yellow yolk, exhibiting a strong adhesive chorion (Figure 1). Each spawning event produced an average of 66.5 ± 2.43 eggs, with an average diameter of 3.896 ± 0.022 mm. No unfertilized eggs were observed, indicating that there are no reproductive problems. Embryonic development is illustrated in Figure 1.
Embryonic and larval ontogeny of Dekeyseria picta, showing development from 0 days after fertilization (DAF) to 15 days after hatching (DAH). Chorion (Ch); head(H); heart (Ht); somites (S) yolk sac (V); tail (T). Scale bar 1 mm.

The duration of embryonic development ranged from three to seven days. However, the average hatching time for D. picta was observed to be 3 days post-fertilization (DAF), with larval development completed by day 15. In the following, we present observations from a single spawning event, for which the approximate time of reproduction was known, and developmental progress was monitored up to 15 days after hatching (DAH).
The stages from the zygote to the differentiation of embryonic germ layers occur within the first six hours (Figure 1A). After the first DAF, somitogenesis and tail release occurred, the notochord was established, and the cranial and caudal regions became distinct (Figure 1B). Somites were visible, and the onset of the heartbeat was detected alongside observed muscle contractions (Figure 1 B–C). At the hatching stage, the perivitelline space was significantly reduced, and muscle contractions intensified (Figure 1D). After hatching, the larvae depended on yolk sac reserves for their initial development, which significantly decreased by day 6 DAH (Figure 1E–G). At that point, external feeding began, and complete larval development was achieved by day 15 (Figure 1H).
Hatched larvae were categorized into five distinct developmental phases. During all hatching phases, the larvae exhibited open mouths and black pigment spots on the dorsal region of the yolk sac. In phase 1, larvae were transparent and segmented, with well-developed but unpigmented eyes; the swim bladder was clearly visible (Figure 2A). In phase 2, the larvae remained transparent but began to show initial eye pigmentation, marking the early stages of cardiovascular development, including the onset of the heartbeat, along with dorsal pigment spots (Figure 2B). In phase 3, the larvae displayed more advanced cardiovascular development, fully pigmented black eyes, and increased dorsal pigmentation (Figure 2C). Phase 4 saw the embryos becoming even more advanced, featuring distinct eye structures (such as the pupil, iris, and choroid) and pigmentation distributed throughout the body (Figure 2D). Finally, in phase 5, the larvae were significantly more developed, exhibiting a body shape resembling that of loricariids. The yolk sac changed from a round to an oval shape, extending longitudinally along the body, and large pigment patches appeared, resembling the transverse black lines typical of juveniles and adults (Figure 2E).
Newly hatched larvae of Dekeyseria picta at developmental phases 1–5. Panels (A–E) show each phase, with the corresponding days after fertilization (DAF) indicated. Heart (Ht); eye (E); mouth (M); yolk sac (V). Scale bar 1 mm.

The hatching rate was less 40%, likely influenced by variations in chorion rupture efficiency and hatching phase. The process begins with the reduction of the perivitelline space (Figure 3A), followed by the rupture of the chorion (Figure 3B–C), but their attempts to hatch can lead to strangulation and death (Figure 3D).
Embryo of Dekeyseria picta attempting to hatch (A). Panels (B–D) show strangulation (asterisk) caused by the highly elastic and adhesive chorion (Ch). Head (H); tail (T); yolk sac (V). Scale bar = 1 mm.

Discussion
Changes in water parameters are known to directly influence fish reproduction by synchronizing spawning with periods of increased food availability and suitable habitats. This synchronization enhances the survival and growth of offspring (Junk et al., Reference Junk, Bayley and Sparks1989; Wootton and Smith, Reference Wootton and Smith2015; Servili et al., Reference Servili, Canario, Mouchel and Muñoz-Cueto2020; Mignien and Stoll, Reference Mignien and Stoll2024). In this study, the minimal changes in water parameters observed during the breeding season of D. picta suggest that even subtle environmental cues can trigger reproductive events. This highlights the sensitivity of the species to its aquatic environment. These findings offer insight into how the reproductive timing of D. picta may be well adapted to enhance the chances of offspring survival and growth.
The quantity of D. picta eggs was significantly higher than that of other loricariids, such as Hypancistrus zebra (Pereira and Henriques, Reference Pereira and Henriques2019; Viana et al., Reference Viana, Gonçalves, Ferreira, Mendes and Rocha2023) and Hypancistrus yudja (Sousa et al., Reference Sousa, Sousa, Oliveira, Sabaj, Zuanon and Rapp Py-Daniel2025), which typically spawns around 15–20 eggs. The size of D. picta eggs is comparable to that of larger species like Hypostomus ternetzi and Megalancistrus aculeatus, both of which produce eggs approximately 4 mm in diameter (Suzuki et al., Reference Suzuki, Agostinho and Winemiller2000). The variation in egg size can be attributed to differences in parental care and nesting strategies (Suzuki et al., Reference Suzuki, Agostinho and Winemiller2000). The larger size of D. picta eggs, along with their highly elastic chorion, may be linked to the resistance needed to support the guarding behavior of the male. The male uses its enlarged pelvic fins (Silva and Py-Daniel, Reference Silva and Rapp Py–Daniel2018) and employs its body weight to protect the eggs, helping to prevent them from being displaced in fast-flowing waters.
The chorion, which is the outer layer of the egg, serves to shield the embryo from the surrounding aquatic environment and mechanical stress until hatching occurs (Rizzo et al., Reference Rizzo, Sato, Barreto and Godinho2002; Pérez-Atehortúa et al., Reference Pérez-Atehortúa, Hernández Arias and Dantagnan2023). These structural characteristics are common among loricariids and have also been observed in other species, such as Rhinelepis aspera (Perini et al., Reference Perini, Bazzoli, Rizzo and Sato2009), Hypancistrus zebra (Viana et al., Reference Viana, Gonçalves, Ferreira, Mendes and Rocha2023), and Hypancistrus seideli (Reis et al., Reference Reis, Abe, Alves, Oliveira, Viana, Takata and Rocha2025; Viana et al., Reference Viana, Abe, Oliveira, Rocha, Reis and Servili2025). This suggests a potential adaptive trait that enhances egg protection under specific environmental conditions.
In loricarids, the development time can vary between species; for instance, it takes two days for Rhinelepis aspera (Perini et al., Reference Perini, Bazzoli, Rizzo and Sato2009) and five days for H. seideli (Reis et al., Reference Reis, Abe, Alves, Oliveira, Viana, Takata and Rocha2025). However, we report for the first-time differences in embryo development within a the same loricariid species. We identified two distinct strategies that may contribute to the embryonic developmental plasticity of this species.
One of these strategies involves a diapause-like state in which embryos appeared to pause development at phases 1 or 2 without evident utilization of their yolk reserves, as no visible changes in yolk sac size were observed during this period. Although the duration of this pause varied among embryos, occurring between days 4 and 6, the yolk remained visually unchanged until the transition to the subsequent developmental phase. This pause is typically metabolic in nature, leading to reduced energy expenditure, and may be either obligatory or facultative depending on environmental conditions (Wourms, Reference Wourms1972). Diapause happens during specific embryonic stages, involves a significant decrease in metabolic rate, and can vary based on the strategy used to optimize hatching in response to specific environmental factors (Wourms, Reference Wourms1972). Notably, despite these periods of developmental arrest or slowed growth, D. picta embryos remained responsive to external stimuli, reinforcing the idea of a diapause-like state.
Another strategy observed was the potential for retarded hatching, where fully developed embryos stay inside the chorion without hatching, even though they are capable of doing so (Wourms, Reference Wourms1972). In annual fishes, this strategy ensures that fry emerge only when environmental conditions are favorable for survival (Kroll, Reference Kroll1984). However, in D. picta, we believe this phenomenon occurs to a lesser extent, potentially allowing larvae to mature within the protective environment of the egg. This retarded hatching also reflects developmental variability and serves as a bet-hedging mechanism in unpredictable habitats (Wourms, Reference Wourms1972). This adaptability may explain the ability of D. picta to utilize such a strategy, given that hydrological conditions and water parameters can fluctuate rapidly in the river pulses that influence their local environments.
In this study, the hatching rate for D. picta was approximately 40%, which is about half of the rate observed in H. seideli (Reis et al., Reference Reis, Abe, Alves, Oliveira, Viana, Takata and Rocha2025). This difference can be result of the phase of embryo at hatching moment. Hatching can occur at various developmental stages, but D. picta larvae that hatch too early (phases 1–3) often do not survive. This is primarily because the embryos struggle to overcome the strong elasticity and adhesiveness of the chorion. In loricariids, adhesive eggs are encased in a thick gelatinous chorion that enhances survival by protecting the clutch (Rizzo et al., Reference Rizzo, Sato, Barreto and Godinho2002). For D. picta, the chorion offers additional protection in fast-flowing blackwater environments; however, it also presents a challenge for prematurely hatched larvae, preventing early hatching.
Environmental conditions can affect the properties of the chorion and may alter the timing of larval emergence, potentially leading to premature hatching and reduced survival rates (Valdebenito et al., Reference Valdebenito, Figueroa, Valdebenito and Paiva2021). Key factors such as temperature (Thépot and Jerry, Reference Thépot and Jerry2015), conductivity (Mignien and Stoll, Reference Mignien and Stoll2024), and pH (Röpke et al., Reference Röpke, Pires, Zuchi, Zuanon and Amadio2024) directly influence embryonic development. In this study, we were unable to determine the specific conditions affecting hatching time or the exact role of the chorion in facilitating successful emergence. Therefore, it is essential to gain a better understanding of the biochemical composition and structural characteristics of the chorion, as well as the impact of environmental conditions on survival.
Technological interventions such as aquaculture and controlled breeding help conserve understudied Neotropical fish species (Novák et al., Reference Novák, Hofmann, Hohl, Magalhães and Patoka2022). For species like D. picta, which lack reproductive records, developing captive-breeding protocols provides essential baseline data on reproductive biology, early development, and environmental tolerances. These methods support ex situ conservation, reduce pressure on wild populations, and promote sustainable ornamental fisheries (Bertolini et al., Reference Bertolini, Lopez, Nascimento, Arashiro, Silva, Santos, Senhorini and Yasui2020).
In this context, the findings on the embryonic development of D. picta are important. The species can adjust hatching timing through diapause-like and delayed hatching strategies. This flexibility likely helps the species adapt to rapidly changing hydrological conditions and is relevant for conservation and captive breeding. Further research should focus on optimizing incubation and identifying environmental factors that improve hatching success. This will advance aquaculture-based conservation and sustainable use of the species.
Acknowledgements
The authors thank the indigenous fishers from Matavén, Vichada (Colombia), involved in the REDD+ Matavén productive project on ornamental fishes, especially the Piaroa community of La Urbana, for their support in collecting wild D. picta specimens. We used Grammarly (Grammarly Inc.) to assist in improving the English grammar. All content was critically reviewed and verified by the authors.
Competing interests
The authors declare that there is no conflict of interest.
Funding information
This study was financed by the REDD + Matavén project through Mediamos F y M S.A.S., with additional support from Asociación de Cabildos y Autoridades Tradicionales Indígenas de la Selva de Matavén – ACASITEMA and the FUNINDES Colombia Foundation.
Ethical standards
All procedures involving fish were conducted in accordance with Colombian regulations for the use of aquatic organisms in research, under the authorization of the National Authority for Aquaculture and Fisheries (AUNAP), Permit for Scientific Research, Resolution No. 1919 of 2023.