Introduction
Protein turnover refers to the renewal of proteins in a cell, tissue or organism and involves the continuous degradation and synthesis of proteins that do not lead to net changes in protein mass. The protein accretion occurring in growing animals is the result of a greater intensity of protein synthesis than that of protein degradation. In the growing state, the protein turnover rate (amount of replaced proteins per unit of time) equals the total protein degradation or, alternatively, the amount of freshly synthesized protein necessary to replace the amount of degraded protein. The protein turnover in growing ruminants is large compared to the net protein deposition, with as high as 94% of the whole body protein synthesis only serving to counterbalance the protein degradation occurring in fattening young bulls (Lobley, Reference Lobley2003). In addition, this large turnover is accompanied by a high-energy cost for the ruminant, with only protein synthesis accounting for 23% of the total energy expenditure in ruminants (Caton et al., Reference Caton, Bauer and Hidari2000). Nevertheless, this dynamic state represents an essential mechanism for life by enabling maintenance services, such as metabolic regulation, cellular repair and rapid adaptation against environmental changes, among other functions.
Standard methods for whole-body protein turnover (WBPT) assessment are based on either precursor or end-product methods (Waterlow, Reference Waterlow1984) consisting of continuous or single-dose intravenous infusions of stable isotope-labelled amino acids (AAs) and quantification of the labelling in either the free AA precursor pool (plasma) or catabolic end-products (urine). The main drawbacks associated with the evaluation of the protein turnover rate through these standard methods are that they depend on (i) a short-term evaluation (from a few hours [precursor method] to a few days [end-product method]), (ii) an invasive procedure and usually non-physiological conditions, (iii) the requirement of a controlled environment with confined animals and usually steady-state conditions (precursor method) and (iv) expensive methods that preclude its application to a large number of animals. Alternatively, less expensive and less invasive methods have been explored, such as total urinary 3-methyl-histidine excretion (Harris and Milne, Reference Harris and Milne1981), to evaluate whole-body protein degradation. However, the use of 3-methyl-histidine urinary excretion to estimate protein turnover also has drawbacks. These include a relatively short-term evaluation (i.e. usually between 4 and 6 days) that is restricted to myofibrillar muscle protein (myosin-actin) turnover, which is not applicable to sheep or pigs (Nishizawa et al., Reference Nishizawa, Toyoda, Noguchi, Hareyama, Itabashi and Funabiki1979) and is subjected to an accurate estimation of the muscle mass in the body (Castro Bulle et al., Reference Castro Bulle, Paulino, Sanches and Sainz2007).
A new isotopic approach was originally developed in animal ecophysiology (Fry and Arnold, Reference Fry and Arnold1982; Tieszen et al., Reference Tieszen, Boutton, Tesdahl and Slade1983) to model the rate at which animal tissues incorporate the isotopic signature of a new diet in view of accurate food web assessment. This new isotopic approach is currently being applied mainly in marine animal species (Abimorad et al., Reference Abimorad, Ducatti, Castellani, Jomori, Portella and Carneiro2014; Mohan et al., Reference Mohan, Smith, Connelly, Attwood, McClelland, Herzka and Walther2016) to evaluate the metabolic turnover rate of animal tissues. This isotopic method consists of following the dynamic isotopic change (i.e. enrichment or depletion) in animal tissues immediately after a change in the natural isotopic composition of the diet (i.e. diet switch). The rate at which animal tissues will incorporate the isotopic signature of the new diet seems to be mostly driven by their protein turnover rate (Carleton and Martinez del Rio, Reference Carleton and Martinez del Rio2005; MacAvoy et al., Reference MacAvoy, Macko and Arneson2005; Braun et al., Reference Braun, Auerswald, Vikari and Schnyder2013), and some authors suggest that the protein turnover rate might be predicted from isotopic incorporation studies (Carleton et al., Reference Carleton, Kelly, Anderson-Sprecher and Martinez del Rio2008). This approach has already been explored in ruminant tissues (Harrison et al., Reference Harrison, Schmidt, Moloney, Kelly, Rossmann, Schellenberg, Camin, Perini, Hoogewerff and Monahan2011; Bahar et al., Reference Bahar, Harrison, Moloney, Monahan and Schmidt2014) for assessing the time needed for muscles to reflect the isotopic signature of a diet in view of inferring the geographical origin and the feeding system used for meat production (i.e. isotopic dietary reconstruction). However, the isotopic approach used in most ruminant and marine animal studies did not repeat the measures from the same animal, sampled only one tissue per animal and slaughtered individuals at different times (Harrison et al., Reference Harrison, Schmidt, Moloney, Kelly, Rossmann, Schellenberg, Camin, Perini, Hoogewerff and Monahan2011; Abimorad et al., Reference Abimorad, Ducatti, Castellani, Jomori, Portella and Carneiro2014). Thus, these studies only provided information about the turnover of specific sampled tissues and not of the whole animal body. Because most of the nitrogen from animal protein is excreted through urine, our hypothesis is that the urinary isotopic N turnover rate assessed from multi-point sampling from the same animal is a non-invasive proxy of the long-term whole-body fractional protein degradation rate (WBPT in a growing animal in %/day).
Thus, the aim of this study was to adapt the tissue isotopic turnover approach (MacAvoy et al., Reference MacAvoy, Macko and Arneson2005; Abimorad et al., Reference Abimorad, Ducatti, Castellani, Jomori, Portella and Carneiro2014) to ruminant urine samples as a non-invasive proxy of the long-term WBPT in a large number of growing-fattening beef cattle. In addition, we also measured the isotopic turnover of plasma proteins as an indicator of the fractional protein synthesis rate (FSR; in %/h) of plasma proteins. Because no gold standard method is currently available for measuring the WBPT over a long period of time (several months), we evaluated this proxy by assessing its ability to detect differences across two dietary factors known to impact WBPT: (i) the protein content and (ii) the dietary AA profile. In this sense, the dietary protein content has been identified as the most important dietary factor impacting the protein turnover rate (Waterlow, Reference Waterlow2006), while the dietary AA profile is expected to affect the protein turnover rate to a lesser extent according to some cattle studies (Wessels et al., Reference Wessels, Titgemeyer and St Jean1997). For this purpose, we measured the kinetics of isotopic nitrogen (δ 15N) depletion in urine and plasma proteins over a 5-month period following a slight decrease in the δ 15N of the diet of 36 fattening young bulls fed diets formulated at two different protein and methionine contents.
Material and methods
Animals, diets and performance test
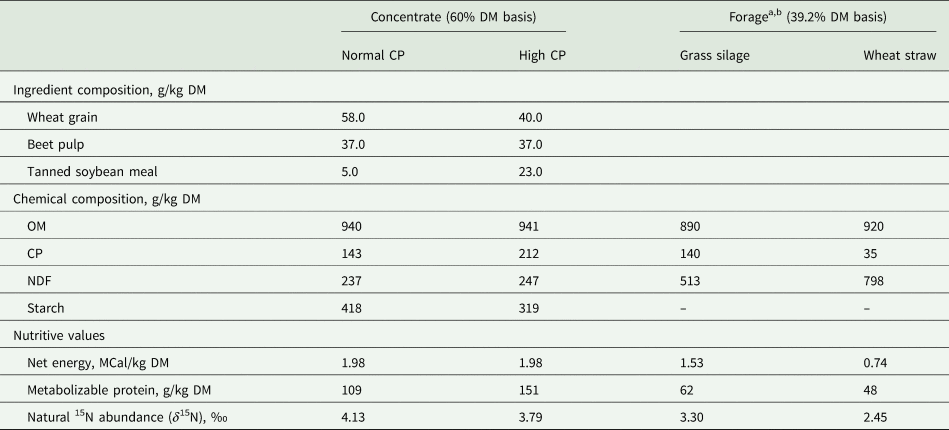
Thirty-six growing-fattening Charolais bulls (320 ± 33 kg and 266 ± 22 days) were assigned to one of the four experimental diets (n = 9/treatment) resulting from a factorial 2 × 2 design: two dietary metabolizable protein levels (100% [Normal] v. 120% [High] of the requirements; INRA, 2018) crossed with two dietary methionine contents (unbalanced diet [2.0 g Met/100 g metabolizable protein] v. balanced diet [2.6 g Met/100 g metabolizable protein]). All diets were iso-NE per kg DM and formulated at a forage-to-concentrate ratio of 60:40. The amounts of feed distributed were adjusted daily to ensure at least 10% refusals. Balanced and unbalanced diets were identical in feed and chemical composition within each dietary CP level and only differed in the supplementation with rumen-protected methionine (7 g/day/animal of Smartamine®, Adisseo) in balanced diets. The concentrate feed composition and chemical composition of the concentrates and forages are shown in Table 1. Animals were housed indoors in free stalls equipped with electronic gates (Dairy gate®, EFEI, Villeroy, France) to measure individual daily feed intake. Water was available ad libitum.
Ingredient and chemical compositions of concentrates and forages

a Bicarbonate and trace minerals and vitamins were added into the TMR at proportions of 0.6 and 0.2% on a DM basis, respectively.
b The forage portion of the TMR consisted of 90% grass silage and 10% wheat straw.
Dietary isotopic N switch
The method applied here to assess the WBPT was based on the rate at which tissues and animal N pools incorporate a new dietary 15N isotopic signature following a dietary isotopic switch (Carleton and Martinez del Rio, Reference Carleton and Martinez del Rio2005). However, because the range of natural 15N abundance values (δ 15N; 15N/14N ratio deviation from the international standard [atmospheric N2]) in ruminant feed remains quite narrow (between 0 and 5‰ on average, according to our experience [Cantalapiedra-Hijar et al., Reference Cantalapiedra-Hijar, Ortigues-Marty, Sepchat, Agabriel, Huneau and Fouillet2015]), we created an artificial dietary isotopic switch by incorporating exogenous 15N-labelled urea into the diet as previously reported (Bahar et al., Reference Bahar, Harrison, Moloney, Monahan and Schmidt2014). Once degraded into 15N-ammonia and taken up by rumen microorganisms, 15N-urea enriches animal tissues through the absorbed microbial 15N-AA. The results from a preliminary trial aiming to define the conditions for implementing this method in ruminants showed that for a given animal, the fraction of 15N-urea bypassing directly to urine, without being first incorporated into microbial proteins, was highly variable across time and individuals and led to problems for fitting the progressive urinary 15N-enrichment post-diet switch (data not shown). Thus, we decided to evaluate the animal 15N turnover rates during depletion (Abimorad et al., Reference Abimorad, Ducatti, Castellani, Jomori, Portella and Carneiro2014) rather than enrichment (Bahar et al., Reference Bahar, Harrison, Moloney, Monahan and Schmidt2014) phase. For this, animals were progressively enriched with 15N over 35 days while adapting to their respective diets; each animal received a capsule (10 × 3 mm) daily, in the morning (0830), containing 20 mg of 15N-labelled urea (98% APE; Sigma–Aldrich, St. Louis, USA). This amount of 15N-labelled urea and time was chosen for enhancing the urinary 15N between 10 and 15‰ above that of the basal diet according to the results obtained from a preliminary trial. The capsule was mixed with approximately 200 g of concentrate (the one assigned to the animal) in a small bucket within the feeder just before the only meal distribution (09.00 a.m.). Twenty minutes after administration, it was systematically checked that the capsule had been swallowed by the animal. Less than 5% of capsules were administered by hand directly in the mouth when animals did not swallow it within the first 20 min. The rest of the diet was then distributed to the feeder. On day 36, animals no longer received 15N-labelled urea, and blood and urine were sampled from that day (day 0) onwards.
Sampling and 15N analysis
The time points for sampling both blood and urine were concentrated in the period immediately following the diet switch when isotopic changes are most rapid (Carter et al., Reference Carter, Bauchinger and McWilliams2019). Blood was sampled at 09.00 a.m. by venipuncture from the caudal vein of all animals on days 0, 3, 7, 11, 15, 21, 35, 49, 78 and 141 (n = 10 per animal) after stopping 15N-labelled urea administration (day 0 refers to 24 h after the last 15N-urea administration). Blood was collected into 9 ml evacuated tubes (BD vacutainer, Plymouth, UK) containing lithium heparin as an anticoagulant, centrifuged within the first hour at 2500 g for 15 min at 4°C and stored at −20°C for the determination of δ 15N values in total plasma proteins as previously described (Cantalapiedra-Hijar et al., Reference Cantalapiedra-Hijar, Ortigues-Marty, Sepchat, Agabriel, Huneau and Fouillet2015). Urinary spot samples were obtained from all animals between 09.00 a.m. and 10.00 a.m. on days 0, 1, 2, 3, 4, 7, 9, 11, 14, 17, 35, 70 and 142 (n = 13). For urinary sampling, animals were head blocked for 1 h while eating in the morning, and a bucket (30 × 30 × 15 cm) was placed around the penis through two elastic ropes knotted on the back of the animal. Most animals urinated during the first hour, and only a few samplings were conducted beyond the first hour and always within the first 3 h. Twenty millilitres of urine was then transferred into a tube containing 1 ml of 30% H2SO4 and filtered later in the laboratory through 30 μm standard filter paper to remove fine particles. Filtered and acidified spot urine samples were stored at −20°C before the determination of δ 15N values. Freeze-dried plasma proteins and liquid urinary samples pipetted onto nitrogen-free absorbent (chromosorb) were weighed in tin capsules and analysed for stable N isotope composition (δ 15N) by using an isotope-ratio mass spectrometer (Isoprime, VG Instruments, Manchester, UK) coupled to an elemental analyser (EA Vario Micro Cube, Elementar, Germany). Tyrosine was used as an internal standard and included in every run to correct for possible variations in the raw values determined by the mass spectrometer. The results were expressed using the delta notation.
Isotopic turnover rate modelling and statistical analysis
The post-diet switch δ 15N kinetics measured in each pool (plasma protein and urine) were carefully analysed according to Martinez del Rio and Carleton (Reference Martinez del Rio and Carleton2012) by testing whether they obey 1st-order or higher-order (2nd-order) kinetics according to the following mono- and bi-exponential models, respectively:


where t (d) is the time since the 15N diet switch, δ 15N(t) (‰) is the δ 15N value of the pool at time t, δ 15N0 (‰) is the initial δ 15N value of the pool and δ 15N∞ (‰) is the asymptotic value of the pool after the animal has reached isotopic steady state with its basal diet (without 15N-urea administration). In the mono-exponential model, k (d−1) is the fractional isotopic turnover rate of the pool, while in the bi-exponential model, k 1 and k 2 (d−1) are two distinct fractional isotopic turnover rates, and p and (1–p) are their respective contributions to the whole isotopic turnover.
To determine whether a mono-exponential model was sufficient to adequately fit the δ 15N kinetics, we used the reaction progress variable approach (Cerling et al., Reference Cerling, Ayliffe, Dearing, Ehleringer, Passey, Podlesak, Torregrossa and West2007; Martinez del Rio and Carleton, Reference Martinez del Rio and Carleton2012) based on the rearrangement of equation (1) to yield:

where (1–F) measures the remaining δ 15N distance to the new equilibrium as a proportion of the total isotopic distance between the initial and asymptotic δ 15N value. As illustrated in Appendix S1, we decided which model was required on the basis of a visual inspection of a plot of ln(1–F) against time, depending on whether ln(1–F) was a decreasing linear function of time with slope equal to -k (mono-exponential model) or a sequence of two lines of increasingly shallow slopes equal to –k 1 and –k 2 (bi-exponential model). This graphical analysis was further supported by the Akaike information criterion, where lower values indicate a superiority of one model over another.
To model the effect of the experimental dietary factors on isotopic decay, we followed recommendations by Pinheiro and Bates (Reference Pinheiro, Bates, Chambers, Eddy Hardle, Sheather and Tierney2000) on non-linear mixed-effect models, taking into account the correlation among observations from the same animal. The first step to find the best model structure consisted of obtaining separate fits for each animal through fixed non-linear models according to equations (1) for plasma proteins and (2) for urine, as previously described. This was performed by the nlsList function in R software (nlme package; Pinheiro and Bates, Reference Pinheiro, Bates, Chambers, Eddy Hardle, Sheather and Tierney2000). Then, by examining the individual fits, it was decided which coefficients seemed to vary between animals and thus deserved to be modelled with a random animal effect. Because there was a large between-animal variability in most model parameters, data were statistically analysed through a non-linear mixed-effect model and fitted by restricted maximum likelihood. In this model, experimental dietary factors (protein content, methionine content and their interaction) were considered fixed effects, and the animal was considered a random effect on all model parameters. To avoid over-parametrization in the most complex model (bi-exponential) and to avoid a failure of model convergence, the random effect of the animal was only considered on those model parameters where significant animal variability was noted through graphical and statistical analysis (Pinheiro and Bates, Reference Pinheiro, Bates, Chambers, Eddy Hardle, Sheather and Tierney2000).
Mixed model equations for plasma and urine isotopic decay were, respectively, as follows:


The fixed effects β 1, β 2, β 3 and β 4 represent the mean values of the parameters in the population of individuals. Dietary factors (protein and methionine content as well as their interaction) were tested on these β parameters. The individual deviations from the mean values are represented by the random effects b 1i, b 2i, b 3i and b 4i, which are assumed to be distributed normally with a mean of 0 and a variance–covariance matrix Ψ. The within-group errors ɛij were assumed to be independently distributed and independent of the random effects.
Significant effects were declared when P ⩽ 0.05, and a trend was considered when 0.05>P < 0.10.
Results
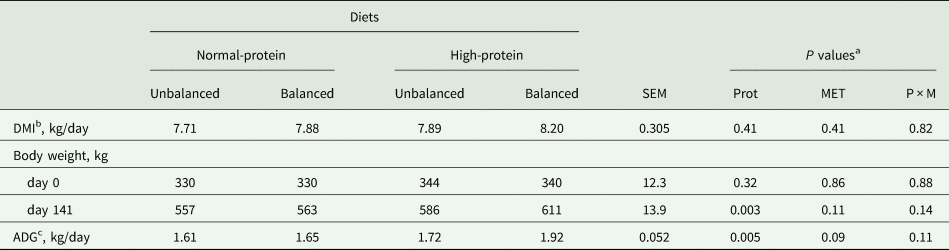
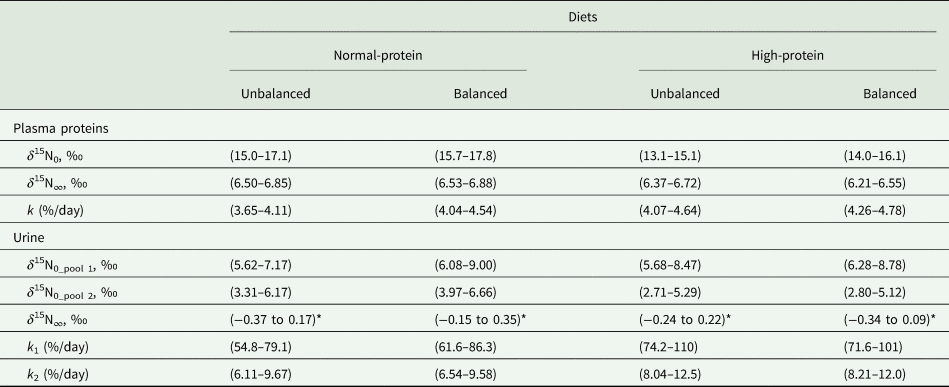
As shown in Table 2, during the length of the applied approach (approximately 5 months), bulls fed high-protein diets had, on average, higher (P = 0.005) daily gains (1.82 kg/day) compared to those fed normal-protein diets (1.63 kg/day on average). On the other hand, methionine-balanced diets tended (P = 0.09), on average, to promote higher daily gains (1.78 kg/day) than those of bulls fed unbalanced diets (1.67 kg/day). No differences in dry matter intake were observed across dietary treatments (P > 0.05). No significant interaction (P > 0.05) between protein level and methionine concentration was observed for any of the variables analysed here. Thus, fitting curves for isotopic decay (Figs 1–4) are presented independently for each of these two experimental factors. Confidence intervals for each parameter estimate are presented in Table 3.
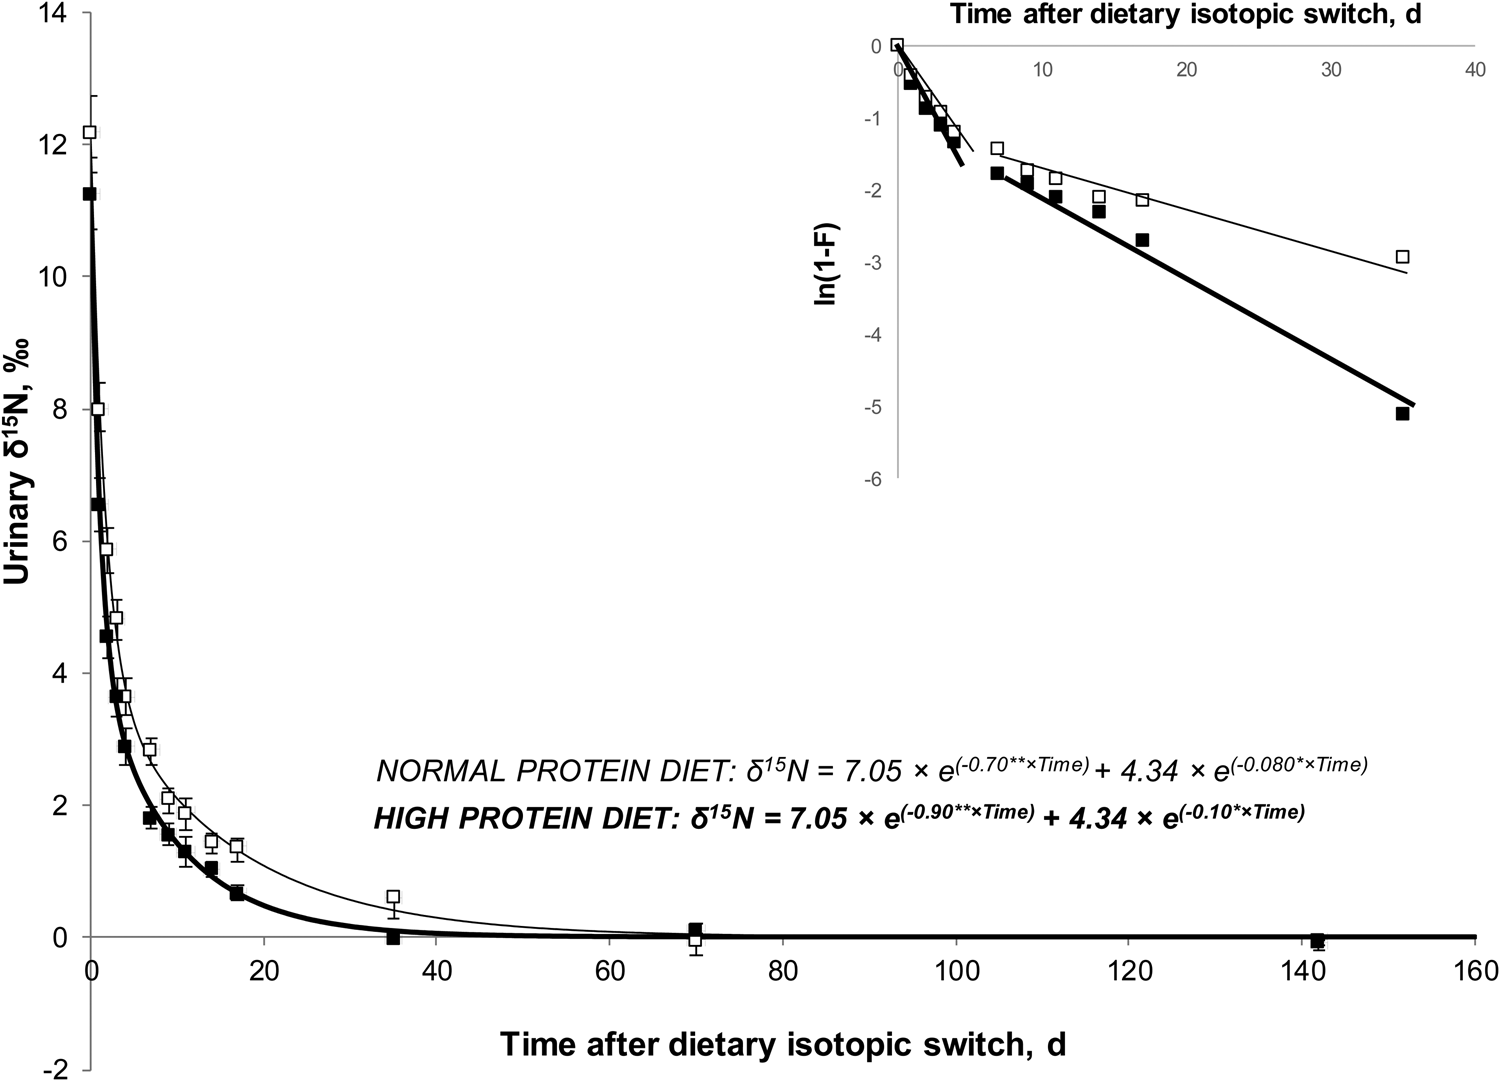
Kinetics of 15N depletion in urine after a 15N diet switch (see Material and methods section) in Charolais fattening bulls fed either normal- (thin line) or high-protein (thick line) diets. Compared to animals fed a normal-protein diet (n = 17), animals fed a high-protein diet (n = 17) showed higher fractional rates of urinary 15N depletion during both the first, rapid (89.9 v. 70.0%/day; P = 0.008) and the second, slow (10.3 v. 8.01%/day; P < 0.001) phases. Inset represents the reaction-progress variable approach [ln(1–F); see Material and methods section] confirming that adequately fitting the 15N-depletion kinetics in urine required a bi-exponential model with two rates for the rapid and slow phases (Martinez del Rio and Carleton, Reference Martinez del Rio and Carleton2012). Significant differences in model parameters across treatments are depicted by asterisks (**P < 0.01; *P < 0.05).

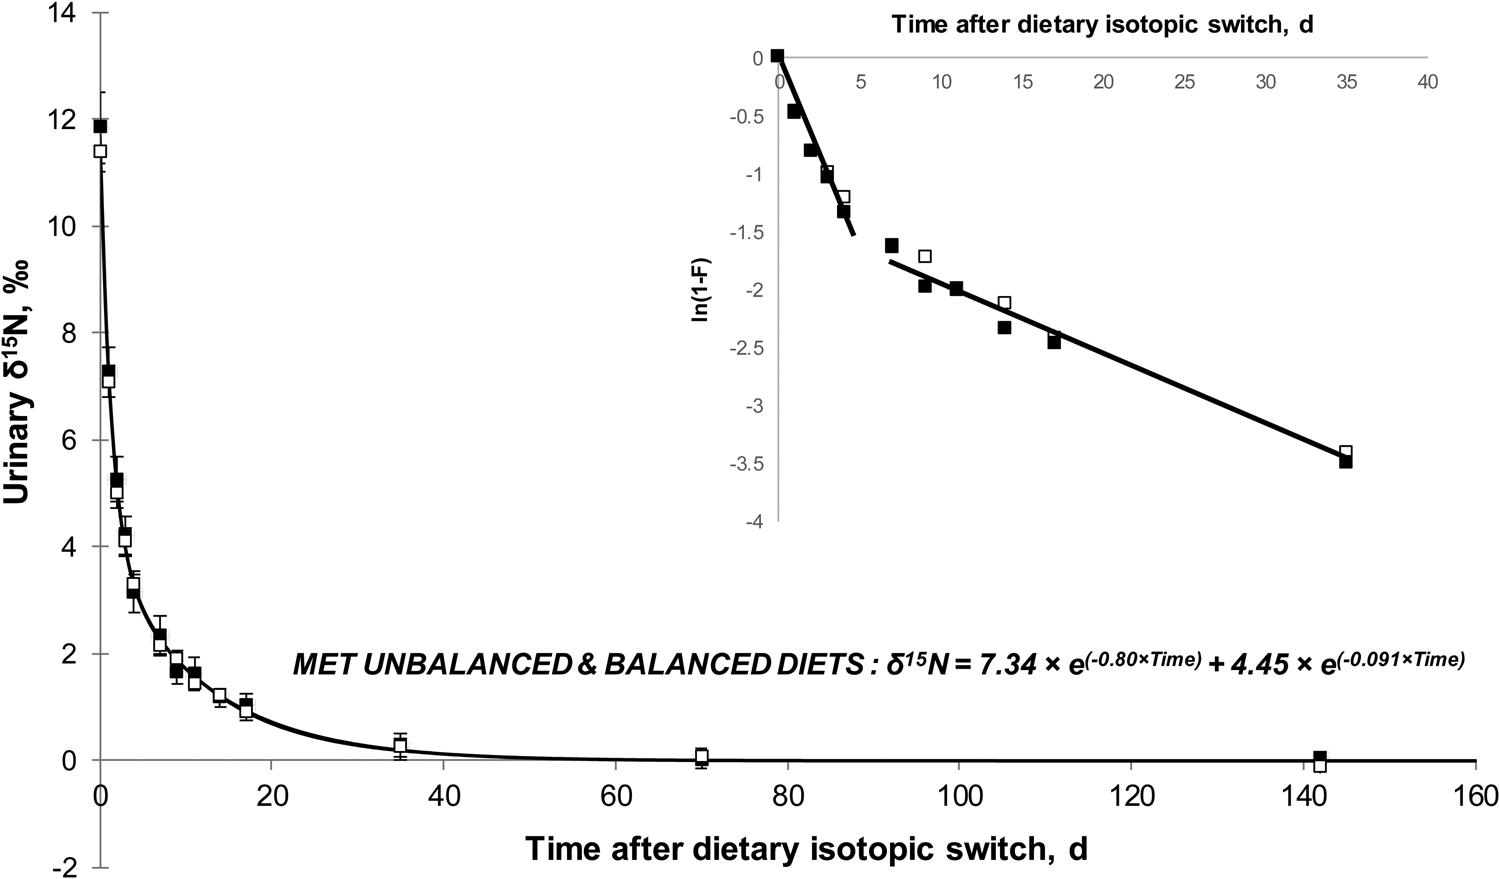
Kinetics of 15N depletion in urine after a 15N diet switch (see Material and methods section) in Charolais fattening bulls fed either balanced (thin line) or unbalanced (thick line) diets in terms of methionine content. Compared to animals fed diets unbalanced in methionine (n = 17), animals fed diets balanced in methionine (n = 17) showed similar fractional rates of urinary 15N depletion during both the first, rapid (80.0%/day; P = 0.92) and the second, slow (9.10%/day; P = 0.80) phases. Inset represents the reaction-progress variable approach [ln(1–F); see Material and methods section] confirming that adequately fitting the 15N depletion kinetics in urine required a bi-exponential model with two rates for the rapid and slow phases (Martinez del Rio and Carleton, Reference Martinez del Rio and Carleton2012).

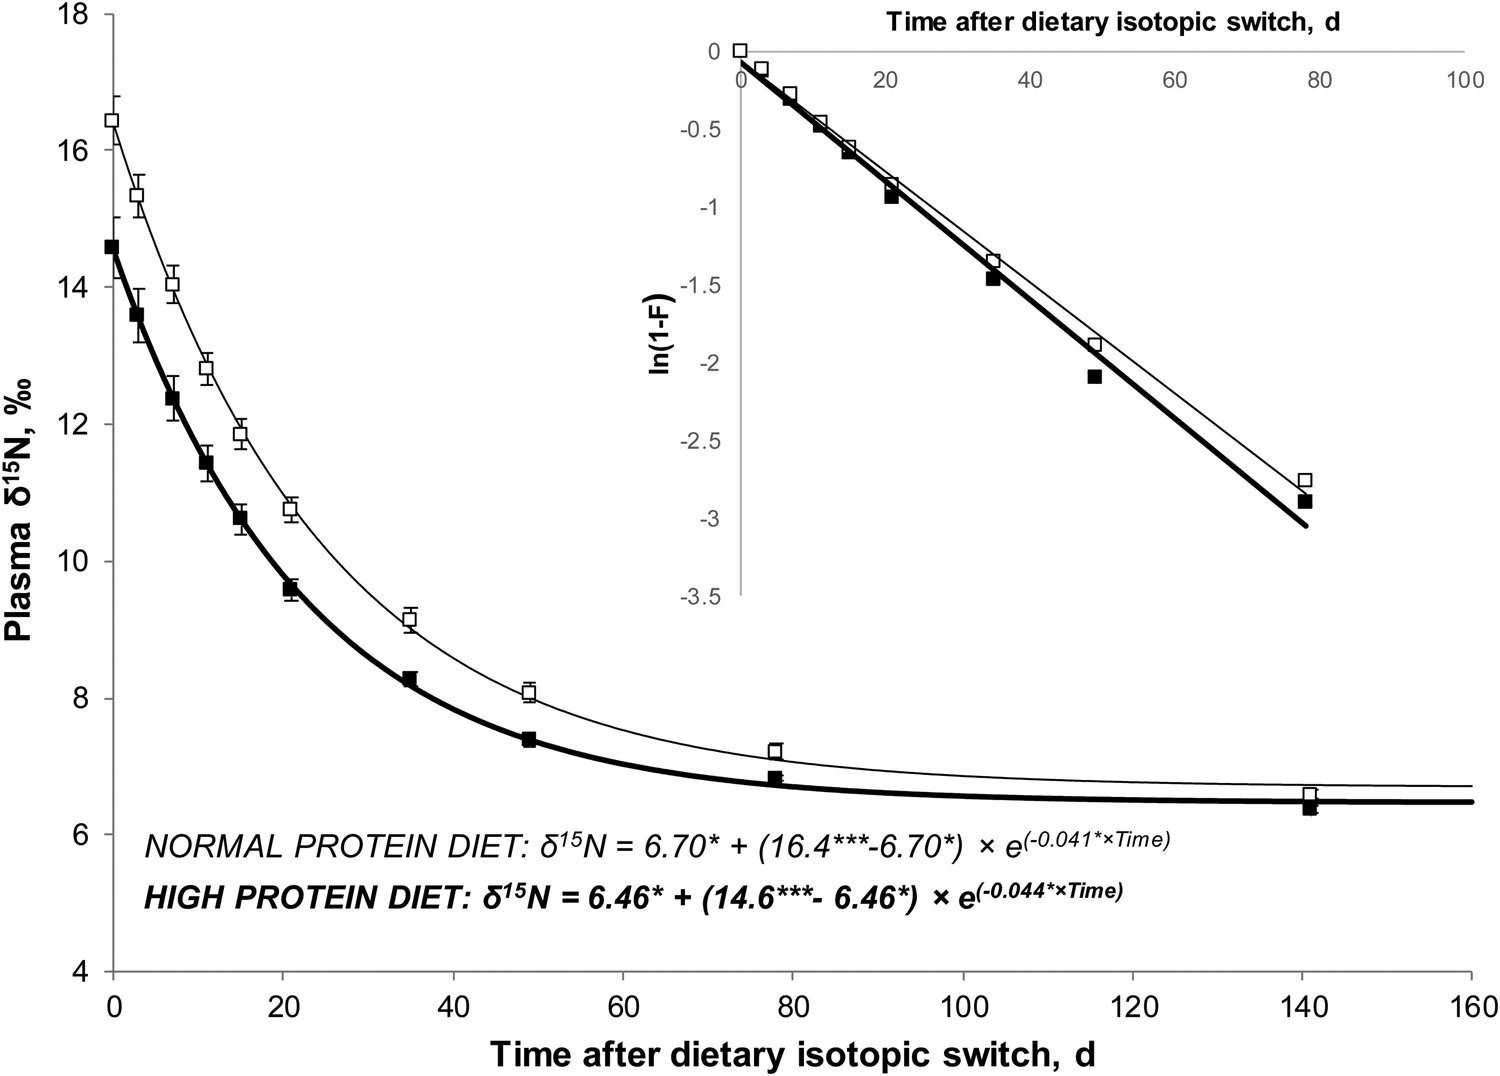
Kinetics of 15N depletion in plasma proteins after a 15N diet switch (see Material and methods section) in Charolais fattening bulls fed either normal- or high-protein diets. Compared to animals fed normal-protein diets (n = 18), animals fed high-protein diets (n = 18) showed lower plasma protein δ 15N values at time 0 (14.6 v. 16.4‰; P < 0.001) and a higher fractional rate of plasma protein 15N depletion (4.42 v. 4.08%/day; P = 0.02). Inset represents the reaction-progress variable approach [ln(1–F); see Material and methods section] confirming that a mono-exponential model was sufficient to adequately fit the 15N-depletion kinetics in plasma proteins (Martinez del Rio and Carleton, Reference Martinez del Rio and Carleton2012). Significant differences in model parameters across treatments are depicted by asterisks (***P < 0.001; **P < 0.01; *P < 0.05).

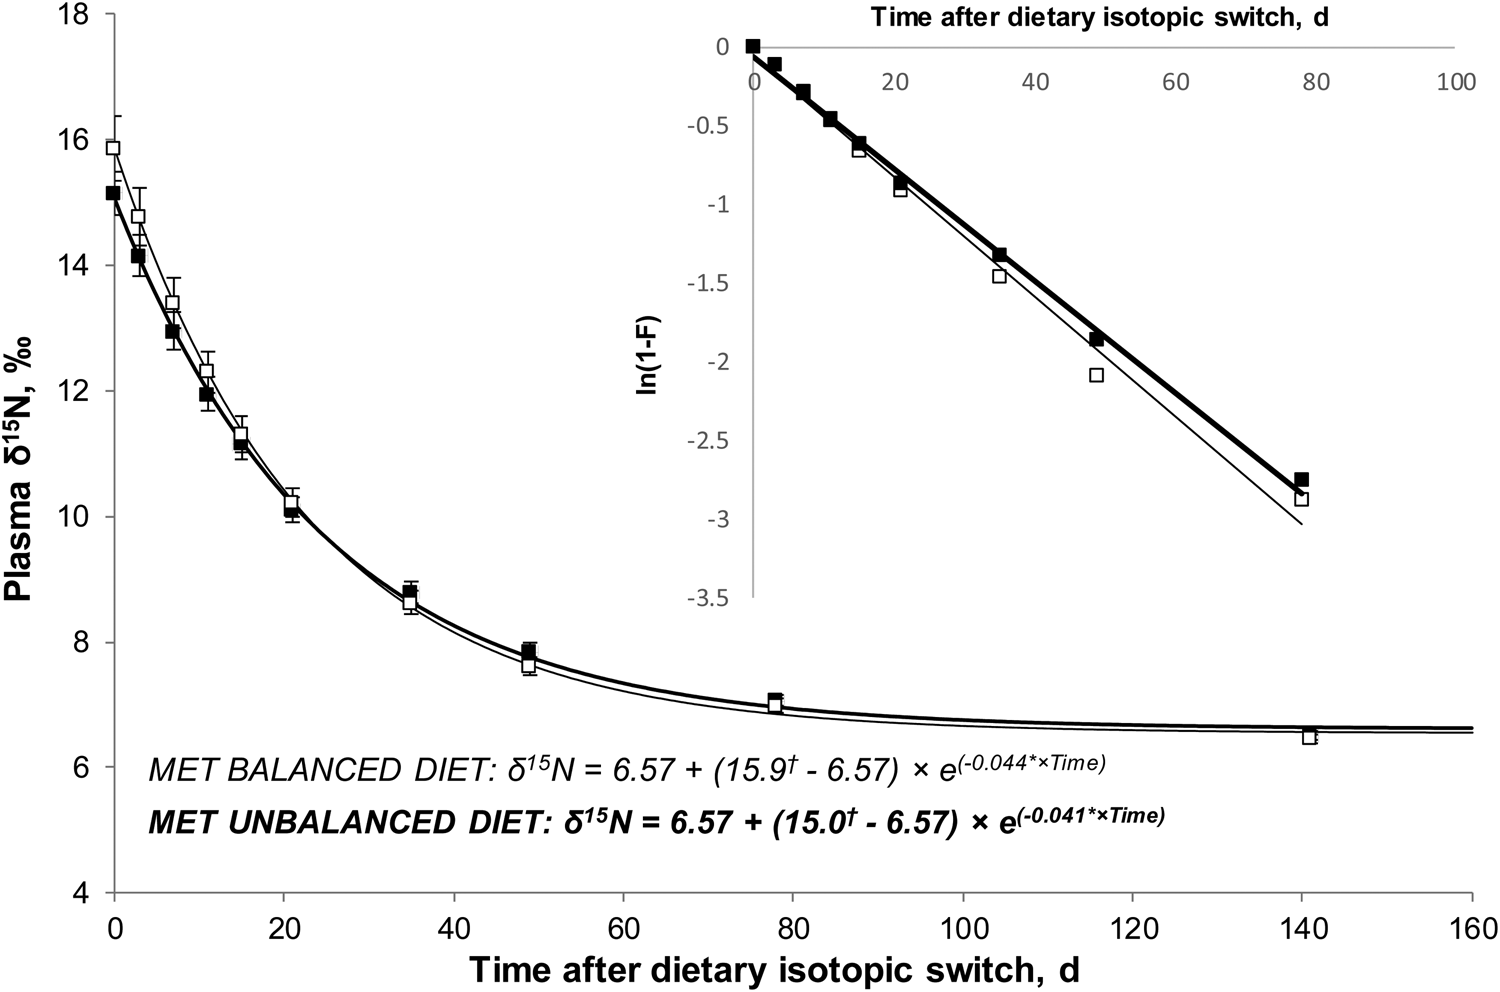
Kinetics of 15N depletion in plasma proteins after a 15N diet switch (see Material and methods section) in Charolais fattening bulls fed either balanced or unbalanced diets in terms of methionine content. Compared to animals fed diets unbalanced in methionine (n = 18), animals fed diets balanced in methionine (n = 18) showed higher plasma protein δ 15N values at time 0 (15.9 v. 15.0‰; P = 0.05) and a higher fractional rate of plasma protein 15N depletion (4.38 v. 4.10%/day; P = 0.05). Inset represents the reaction-progress variable approach [ln(1–F); see Material and methods section] confirming that a mono-exponential model was sufficient to adequately fit the 15N depletion kinetics in plasma proteins (Martinez del Rio and Carleton, Reference Martinez del Rio and Carleton2012). Significant differences in model parameters across treatments are depicted by symbols (†P < 0.10; *P < 0.05).

Animal performance in young Charolais bulls fed diets formulated at two dietary protein levels (normal v. high) and two methionine contents (unbalanced v. balanced)

a Prot: Effect of protein level (normal v. high); Met: Effect of methionine content (Unbalanced v. Balanced).
b Dry matter intake from day 0 to day 141.
c Average daily gain from day 0 to day 141 calculated as the slope of body weight against time.
Confidence intervals (95% CI) of parameter estimates from the isotopic decay curve analysed following an isotopic dietary shift in young Charolais bulls fed the experimental diets

*Estimates not different from 0 (P < 0.05).
Urinary isotopic turnover rate
For δ 15N kinetics in urine, the reaction progress approach clearly identified two independent slopes with a cut-off between day 4 and day 7 (insets in Figs 1 and 2). This demonstrated the existence of two distinct rates of urinary δ 15N depletion after the diet switch and justified the use of a bi-exponential rather than mono-exponential model to adequately fit these data. The individual δ 15N kinetics were indeed correctly fitted for almost all animals (R 2 ≥ 0.96; n = 34) using a bi-exponential model, except for two animals that were badly fitted with no apparent explanation and that were therefore excluded from the analyses. When all data were pooled and analysed through a mixed-effect bi-exponential model, animals fed high-protein diets showed higher values during both the first, rapid (89.9 v. 70.0%/day; P = 0.008) and the second, slow (10.3 v. 8.01%/day; P < 0.001) phases of δ 15N turnover than those of animals fed normal-protein diets (Fig. 1). No effect of methionine content was observed on any model parameter (P > 0.10; Fig. 2).
Plasma isotopic turnover rate
For δ 15N kinetics in plasma proteins, the reaction progress approach showed a single slope (insets in Figs 3 and 4). This demonstrated the existence of a single, homogenous rate of δ 15N depletion in plasma proteins after the diet switch and justified that a mono-exponential model was sufficient for adequately fitting these data. The individual δ 15N kinetics in plasma proteins were indeed correctly fitted (R 2 ≥ 0.98; n = 36) through a mono-exponential asymptotic model. When all data were pooled and analysed through a mixed-effect asymptotic model, lower plasma protein δ 15N values were observed in animals fed high-protein diets than those in animals fed normal-protein diets (Fig. 3) on the first day (δ 15N0; P = 0.04) and at equilibrium (δ 15N∞; P = 0.09). In contrast, diets balanced in terms of methionine content tended (P = 0.09) to have a higher δ 15N value in plasma proteins on day 0 than those unbalanced (δ 15N0 in Fig. 4) but similar δ 15N value (P = 0.47) at equilibrium (δ 15N∞ in Fig. 4). The fractional 15N depletion rate in plasma proteins was higher in animals fed high-protein diets than in animals fed normal-protein diets (4.42 v. 4.08%/day; P = 0.02) and was also higher in those fed diets balanced than in those fed unbalanced diets in terms of methionine (4.38 v. 4.10%/day; P = 0.05).
Discussion
Following a diet change, animal tissues progressively assimilate the isotopic signature of the new diet (Carleton and Martinez del Rio, Reference Carleton and Martinez del Rio2005). The rate at which this occurs is known as the isotopic turnover rate and depends largely on how fast metabolic tissue replacement occurs (Tieszen et al., Reference Tieszen, Boutton, Tesdahl and Slade1983; Arneson et al., Reference Arneson, MacAvoy and Basset2006). We adapted the tissue isotopic turnover approach, extensively explored by ecologists (Martinez del Rio and Carleton, Reference Martinez del Rio and Carleton2012), to the case of ruminant urine and plasma proteins to evaluate the WBPT (protein turnover in a growing animal) over a long period of time (5 months) and the FSR of plasma protein, respectively, in 36 growing-fattening cattle. This isotopic approach is simple to set up and relatively inexpensive (estimated to be <300 dollars per bull), allowing for measurements to be obtained over long periods of time (several months) and without perturbing animals (unlike classic tracer methods with invasive procedures under non-physiological conditions). Although the mechanistic interpretation of isotopic turnover rates is always a complex issue (Martinez del Rio and Anderson-Sprecher, Reference Martinez del Rio and Anderson-Sprecher2008), it is proposed that the rates at which urine and plasma proteins are progressively 15N-depleted following an isotopic diet switch represent non-invasive (or minimally invasive) proxies of the long-term WBPT and plasma protein FSR, respectively. Such proxies could be very useful for future studies on feed efficiency (protein turnover as an energy-consuming process), animal robustness (protein turnover as a maintenance service) and meat quality (in vivo protein turnover associated with the rate of post mortem proteolysis and thus meat tenderness) carried out on a large number of animals.
Biological meaning of isotopic turnover rates
The simplicity of the method described here may contrast with the need to address some methodological considerations for interpreting our results. The rate at which animal tissues will incorporate the isotopic signature of a new diet seems to be mostly driven by their protein turnover rate according to many previous reports (Carleton and Martinez del Rio, Reference Carleton and Martinez del Rio2005; MacAvoy et al., Reference MacAvoy, Macko and Arneson2005; Braun et al., Reference Braun, Auerswald, Vikari and Schnyder2013). Moreover, this has been confirmed by mechanistic models (Martinez del Rio and Carleton, Reference Martinez del Rio and Carleton2012; Poupin et al., Reference Poupin, Huneau, Mariotti, Tomé, Bos and Fouillet2012), demonstrating that the main driver determining the rate of assimilation of the new dietary 15N into a tissue after a diet switch is the protein FSR of that tissue. Thus, the isotopic turnover rate we found in the plasma protein pool (i.e. the k model parameter; Figs 3 and 4) represented a 5-month-averaged FSR (i.e. the sum of 5-month-averaged fractional degradation rates and fractional growth rates, which are supposed to vary with age) and may be proposed as a way to indirectly evaluate the liver FSR of plasma proteins. In contrast, to the best of our knowledge, the isotopic turnover rate of urine has never been analysed mechanistically, and as further discussed, its biological meaning is mostly ascribed to the WBPT and is not directly affected by changes in the whole body protein growth rate. However, some considerations and assumptions need to be discussed to support our biological interpretation.
First, the urinary δ 15N kinetics post-diet switch reflected not only the N metabolism of the animal but also that of its symbiotic rumen microbiota. Because the rumen microbiota contributes to the supply of N compounds to the host (mainly AAs but also purine derivatives), urine would progressively also contain a fraction of the previously 15N-enriched rumen microbiota. However, this would quantitatively have a short-term impact on urinary δ 15N kinetics due to the high protein turnover rate of rumen microbiota (127–686%/day in rumen bacteria; Wallace and McPherson, Reference Wallace and McPherson1987). Second, because of the complex and extensive urea recycling in ruminants, we should not exclude the fact that the clearance rate of the previously administered 15N-labelled urea from the whole body after stopping its administration might contribute, to an undetermined extent, to the urinary 15N depletion rate during the first few hours. In this sense, it has been demonstrated in beef cattle that most infused 15N-labelled urea is excreted through urine within the first 48 h (Wessels et al., Reference Wessels, Titgemeyer and St Jean1997), so its impact on the urinary 15N depletion rate would be very short. Third, we cannot exclude that differences in N absorption, and thus in urinary N excretion, expected across diets (normal- v. high-protein diets) might contribute to the observed differences in the urinary 15N depletion rate. Indeed, the dietary N influx into the plasma pool, while being much smaller than the endogenous AA influx by protein degradation (Lobley, Reference Lobley2003), had the largest δ 15N difference with the endogenous AAs at the beginning of the diet switch (dietary AAs were largely 15N-depleted compared to the endogenous AAs previously 15N-enriched during the administration of 15N-labelled urea). As a consequence, the urinary δ 15N kinetics were probably mainly driven by the dietary AA influx during the first phase (k 1 phase) before being mostly driven by the endogenous AA influx released from whole-body protein degradation thereafter (k 2 phase). Fourth, because the whole animal body was not completely at isotopic steady-state just before the isotopic diet switch (only 35 days of isotopic equilibration were conducted), an overcontribution of the fastest turn-over pools to the first phase of the urinary isotopic decay cannot be ruled out. These four factors (rumen microbiota metabolism, isotopic-labelled urea clearance rate, differences in N absorption across treatments and lack of a real isotopic steady state before the diet switch) would thus have a limited, short impact on the urinary 15N turnover rate during the first, rapid phase (k 1). We proposed that the 15N depletion rate in urine during the second, slow phase (k 2) was mostly driven by the release rate of endogenous 15N-labelled AAs from the degradation of previously labelled endogenous proteins. This progressive release of previously labelled AAs translated first into the free plasma AA pool and then into the urea-N pool resulting from their catabolism. Therefore, we assumed that the urinary 15N depletion rate during the second, slow phase (k 2) was mostly the consequence of the WBPT, whereas the rate during the first, rapid phase (k 1) was likely a mix from the previously evoked mechanisms together with (to some undetermined extent) the protein degradation rate of some very fast turn-over animal N pools.
A limitation to our interpretation could be that some N-containing compounds in urine are metabolically unrelated to protein degradation and AA oxidation. This could represent a potential issue, particularly in ruminants, where urinary urea-N excretion, the main urinary nitrogenous component, may originate, to a high extent, from rumen ammonia production (INRA, 2018) and thus from nitrogenous compounds unrelated to protein degradation and AA oxidation. It can be acknowledged that our modelled k 2 likely integrates the outflow rate of minor urinary nitrogenous compounds not related to AA oxidation and with an endogenous (animal) origin (e.g. creatine, creatinine, endogenous purine derivatives, 3-methylhistidine and other free AAs). Such endogenous nitrogenous compounds were likely previously labelled during 15N urea administration and progressively released from the animal through the urine. However, it should be stressed that (i) the contribution of endogenous nitrogenous compounds to total urinary N remains relatively modest in high-production animals (0.05 g N/kg BW/day; INRA, 2018) and (ii) for some of these nitrogenous compounds, their release rate is closely related to the protein turnover rate (e.g. 3-methyl-histidine as an index of muscle protein degradation and endogenous purine derivatives from nucleic acid turnover rate).
For those urinary nitrogenous compounds not related to AA oxidation and with a ruminal origin (mostly purine derivatives [allantoin and uric acid], hippuric acid and rumen ammonia that has largely transformed into urea), it can be argued, as previously mentioned, that they would probably impact the first, rapid phase of the urinary 15N depletion rate (k 1), but as long as the plasma absorption of such compounds remains relatively constant across time, they will not have an effect on the second, slow phase of this depletion (k 2). Taken together, we can consider that even if k 2 does not strictly correspond only to the WBPT, it may qualitatively reflect this flux and can be proposed as a proxy to evaluate WBPT.
Finally, we recognized that the proposed approach based on isotope decay rates may be problematic for obtaining a real and accurate estimation of WBPT because of the phenomenon of AA reutilization (i.e. the reincorporation of labelled AAs released by protein degradation during protein re-synthesis). Indeed, because overall rates of protein turnover markedly exceed the rates of dietary protein intake, much of the AA substrates for protein synthesis are derived from protein degradation (Lobley, Reference Lobley2003). However, even if AA re-utilization could impact the 15N values at each time point of isotopic decay, we assume that a higher protein turnover (also associated with a higher AA reutilization) will always have a higher k 2 than that of a low protein turnover rate. Thus, for comparing treatments (or even individuals) in terms of WBPT, this approach can still serve as a proxy.
To evaluate the aforementioned biological interpretations, we tested the ability of our method to detect differences across two dietary factors, protein content (normal v. high) and AA profile (diets balanced v. unbalanced in terms of methionine), known to impact the WBPT rate to different extents.
Isotopic turnover rates across dietary factors that impact protein metabolism
Dietary protein content determines the dietary AA flux to the organism and is the major dietary determinant of WBPT rates in humans (Waterlow, Reference Waterlow2006) and farm animals (Lobley, Reference Lobley2003) through the action of catabolic and anabolic hormones. In the present study, the urinary 15N depletion rates during both the first, rapid (k 1) and second, slow (k 2) phases increased, on average, by approximately 28% when the metabolizable protein content was increased by 20%. This finding is in line with the expected increases in dietary AA influx and WBPT with high-protein diets (Waterlow, Reference Waterlow2006) that have been well recorded in k 1 and k 2, respectively. When a similar diet switch approach was applied to adult rats fed diets at or much above the protein requirements (10 v. 30% CP), the urinary turnover rate of 15N increased more than twofold, which was in agreement with an expected higher protein turnover rate (Braun et al., Reference Braun, Auerswald, Vikari and Schnyder2013). Our values for the WBPT (average k 2 = 9.1%/day) are, however, higher than those reported in the few studies using standard isotopic methods in growing ruminants, which themselves encompass a wide range (3.88–8.00%/day whole-body protein FSR in growing heifers [Lobley et al., Reference Lobley, Milne, Lovie, Reeds and Pennie1980]; 6.15–7.63%/day WBPT in growing lambs [Liu et al., Reference Liu, Lobley, MacLeod, Kyle, Chen and Ørskov1995]; calculated WBPT rate of approximately 1.8%/day in growing steers [Wessels et al., Reference Wessels, Titgemeyer and St Jean1997]) but are still lower than other estimates (19.7%/day WBPT rate in growing lambs [Davis et al., Reference Davis, Barry and Hughson1981]). Although the methods are not comparable due to differences in time scales, our higher values compared to those of other cattle studies (Lobley et al., Reference Lobley, Milne, Lovie, Reeds and Pennie1980; Wessels et al., Reference Wessels, Titgemeyer and St Jean1997) could be the consequence of using a late-maturing breed with high growth rates (1.70 kg/day on average for the studied period) that retain between 35 and 45% of their energy as protein (Geay and Robelin, Reference Geay and Robelin1979). The obtained values will need further confirmation and interpretation.
We also found that the plasma protein 15N depletion rate (k) increased with increasing dietary protein content, supporting the idea of greater protein metabolism at all body levels, as revealed through the analysis of urine. Likewise, Tsahar et al. (Reference Tsahar, Wolf, Izhaki, Arad and Martinez del Rio2008) also found in birds that the 15N turnover rate in plasma doubled (from approximately 11 to 20%/day) when the dietary protein shifted from 7 to 16% CP. The impact of dietary protein content on the protein turnover rate of plasma proteins was demonstrated in the 1950s through a study by Steinbock and Tarver (Reference Steinbock and Tarver1954), who injected plasma from donor rats in which the proteins were previously labelled with [35S] methionine into other rats. However, this effect was not observed in ruminants through standard isotopic methods, where the plasma protein FSR remained unchanged in dairy cows fed different dietary metabolizable protein contents (Raggio et al., Reference Raggio, Lobley, Berthiaume, Pellerin, Allard, Dubreuil and Lapierre2007) or sheep undergoing a shift between the fasted to fed state (Connell et al., Reference Connell, Calder, Anderson and Lobley1997). The short-term evaluation inherent to standard isotopic methods together with slow protein synthesis rates of plasma proteins in ruminants (around 6.7%/day; Raggio et al., Reference Raggio, Lobley, Berthiaume, Pellerin, Allard, Dubreuil and Lapierre2007) may explain these results.
On the other hand, no changes in the rate at which urine was progressively depleted in 15N following an isotopic diet switch were found between balanced v. unbalanced diets in terms of methionine content. In contrast, the plasma protein 15N-depletion rate slightly increased, indicating that the protein FSR was enhanced for plasma proteins and, likely, also in other parts of the body. Our findings may indicate that the observed trend of Met-balanced diets improving beef cattle performances (Cantalapiedra-Hijar et al., Reference Cantalapiedra-Hijar, Bahloul, Chantelauze, Largeau, Khodorova, Fouillet and Ortigues-Marty2018) could stem from increased whole-body protein synthesis rather than from a reduction in whole-body protein degradation.
Conclusions
We proposed that the rate at which animal urine is depleted of 15N after stopping the administration of 15N-labelled urea in the diet (i.e. isotopic turnover rate after a diet switch) can be utilized as a non-invasive and simple proxy to evaluate the WBPT rate over a long period of time in a large number of animals. Further studies are warranted to explore the potential and limits of this new promising isotopic approach for evaluating protein turnover. Specifically, future works should evaluate the impact of AA reutilization and urea-N recycling on the N isotopic dynamics in urine and tissues after a diet switch.
Supplementary material
The supplementary material for this article can be found at https://doi.org/10.1017/S0021859620000118
Acknowledgements
The authors would like to thank Vincent Largeau and the staff of Herbipôle for their great technical assistance during this experiment.
Financial support
INRAE's Phase department is acknowledged for supporting the pilot study that served to establish the conditions of the experiment presented here. Adisseo is acknowledged for financially supporting this study.
Conflict of interest
L.B. is employed by Adisseo France SAS, which commercializes Smartamine used in this experiment. The remaining authors declare that the research was conducted in the absence of any commercial or financial relationship that could be construed as a potential conflict of interest.
Ethical standards
The experiment was conducted at Herbipôle (Inra, UE 1414, Theix, France) in compliance with the National Legislation on Animal Care. The C2EA-02 Animal Research Ethics Committee (Auvergne, France) prospectively approved this research, and thereafter, the Ministry of Agriculture (France) validated it with approval number #7180-2016101016361277v4.