1. Introduction.
The Modern Synthesis precipitated the now widely held view that “species evolve as cohesive entities held together by gene flow” (Morjan and Rieseberg Reference Morjan and Rieseberg2004, 1341). This view is crucial to a range of other views in philosophy and biology. For example, it underwrites arguments for a number of popular definitions of ‘species’, including the biological species concept, and it features in arguments for the influential thesis that species are individuals. Nevertheless, I shall argue that there are neglected empirical reasons for rejecting the species cohesion by gene flow view, which I also call The View.
The basic idea is that empirical data shows gene flow is neither necessary nor sufficient for species cohesion. On a number of occasions, Ereshefsky has briefly pointed to this objection (Reference Ereshefsky1988, 429; Reference Ereshefsky1991, 90), but neither thoroughly developed nor straightforwardly endorsed it (e.g., Reference Ereshefsky1988, 429). Perhaps because of this, authors such as Ghiselin (Reference Ghiselin1997, 102ff.) have quickly dismissed the objection. To show such dismissals are hasty, I first articulate The View (Section 2), then discuss its relevant historical aspects (Section 3). This brings needed clarity to The View and helps reveal its philosophical dimensions, but also suggests that many philosophers and systematists have neglected empirical data most relevant to it. These data are latent in and distributed across studies by population geneticists who seldom explicitly generalize the discussion of their data within the more conceptual context of species cohesion. Thus this paper's main innovation consists in integrating old and new gene flow data and adding a philosophical gloss to those data while bringing them into the context of the species cohesion problem. This strategy affords the arguments for the conclusions that gene flow is neither necessary (Section 4) nor sufficient (Section 5) for species cohesion. In closing, I discuss implications of these conclusions (Section 6).
2. The View.
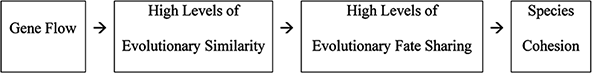
Many biologists and philosophers agree that species are cohesive entities, but then disagree about what is responsible for such cohesion. This is the species cohesion problem, and as a putative answer to it The View implies that species cohesion is a property had by a species in virtue of a particular chain of determination. To unpack this further, consider Figure 1, where each of the crucial phenomena in the chain is listed and arrows are used to simplistically represent the direction of the relations of determination between phenomena. Consider species cohesion first, as I explicate the chain from right to left, against the arrows.
Species cohesion by gene flow.

Roughly, ‘species cohesion’ refers to the evolutionary unity manifest within each species as it travels a distinct trajectory through evolutionary space (Wiley Reference Wiley1981). Species are thus cohesive with respect to evolutionary pressures. The conspecifics that a species comprises tend to face evolutionary pressures, such as selection and drift, as one. As a result, biologists often say that conspecifics tend to share evolutionary fates and that, as Figure 1 implies, species cohesion consists in high levels of evolutionary fate sharing found among conspecifics.
Note it is not that conspecifics always share fates. Variation is inherent within species and consequently conspecific fates vary and evolution is possible; hence, species cohesion is a property admitting of degrees. Neither is it that only conspecifics share fates. Members of distinct species can share evolutionary fates in significant senses; however, conspecifics tend to share fates in ways and to degrees that non-conspecific organisms do not. And although authors famously disagree about what it is that constitutes conspecificity, most imply that the high levels of fate sharing typical of conspecifics owe proximally to high levels of genotypic, phenotypic, and relational similarity (Grant Reference Grant1980; Templeton Reference Templeton, Otte and Endler1989, 3). For example, salamanders in a population of Ensatina eschscholtzii may tend to share grim evolutionary fates during a drought because they tend to lack particular moisture retention genes (genotypic similarity), tend to have thin skins more generally (phenotypic similarity), or because similar relations in which each tends to stand (relational similarity) come to be disadvantageous relations when the drought changes the population-level frequency of certain traits. Figure 1 refers to these kinds of similarity relations as kinds of evolutionary similarity. And in the context of evolutionary pressures, high levels of evolutionary similarity among conspecifics lead to the high levels of fate sharing in which species cohesion consists.
But on The View, such high levels of similarity are not fundamentally responsible for species cohesion, because they in turn owe primarily to gene flow. Roughly, gene flow is transmission of genes from one organism to another. Such transmission is typically realized in one or another form of reproduction, with sexual reproduction being the paradigm case, that is, when organisms mate, genes from each are transmitted to offspring. Authors also often talk of gene flow as “the movement of genes from one population into the gene pool of another” (Futuyma Reference Futuyma1998, 315). This is relevant here because The View implies that species often cohere in the sense that conspecific populations face common selection regimes and then respond similarly because gene flow between them ensures they are sufficiently similar in the eyes of selection. But technically, genes flow from one population to another only when they flow between organisms.
Why think that gene flow is, as Hull puts it, “fundamental in its own right,” such that, “two organisms produce genetically similar organisms because they interbreed,” rather than, “two organisms can be interbred because they are genotypically similar” (Reference Hull1981, 145)? Presumably, the flow of genes, not the genes themselves, is fundamental because such flow distributes genes, which is to distribute important causes of similarity relations in which conspecifics stand. From this, it is inferred that gene flow is the primary manipulator of levels of evolutionary similarity relations within and across conspecific populations. Gene flow then seems primarily responsible for levels of evolutionary similarity relations being high among conspecifics. These high levels then lead, in the context of evolutionary pressures such as selection, to the high levels of evolutionary fate sharing in which species cohesion consists. Hence gene flow is thought ultimately responsible for species cohesion. Notice that the generation of species cohesion thus seems a thoroughly dynamic affair, where gene flow not only ‘homogenizes’ populations, but ‘integrates’ them as well (Grant Reference Grant1980, 157).
Although one might hold that gene flow generates only some instance of species cohesion, The View generally privileges gene flow as an explanans of species cohesion. It treats gene flow as primarily responsible for all or the great majority of cases of species cohesion, with the exception cases being special cases that do not establish wide-spread significance for alternative or additional factors of species cohesion. Some authors support this view by suggesting (usually implicitly) gene flow is necessary (Mayr Reference Mayr1970), or sufficient (Brogaard Reference Brogaard2004), or both necessary and sufficient (Ghiselin Reference Ghiselin1997) for species cohesion. More generally, The View remains entrenched within contemporary biological theory and practice (Futuyma Reference Futuyma1998, 453), despite objections from a few localized research programs. To appreciate how my argument both draws upon and adds to previous objections, let me offer brief historical clarifications.
3. Entrenchment and Neglect.
Despite some interdisciplinary efforts, a certain disciplinary distance has existed between The View as a theoretical or conceptual view of species, and the empirical data most relevant to it. Systematists and philosophers of biology have been the primary discussants of The View, yet experimental population geneticists collect the most salient gene flow data. A gap has grown between theory and data. On one hand, population geneticists tend not to collect and discuss their data within the context of The View, and often uncritically adopt the view as an assumption that underlies their quantitative examinations of gene flow (e.g., Palumbi Reference Palumbi2003; and see Bilodeau et al. Reference Bilodeau, Felder and Neigel2005, 151). In part this is because the research questions population geneticists ask tend, for good reasons, to concern population structure and differentiation rather than the nature of cohesion per se. Thus, data most relevant to The View lies implicit and distributed across a number of population genetics studies.
On the other hand, systematists and philosophers of biology have tended to rely (implicitly at least) on the argument sketched above without consulting all the relevant quantitative data on gene flow that is implicit and distributed in a discipline adjacent to them. They are not entirely at fault. Because many population geneticists themselves, especially through to the 1990s, uncritically adopted The View, they seldom interpreted their data in a way that raised flags for potential interdisciplinary observers (Joseph Neigel, personal communication, November 14, 2005).
Fortunately, a few papers corral relevant empirical studies of gene flow and species cohesion. I will range over these studies, especially those in Ehrlich and Raven's classic Reference Ehrlich and Raven1969 paper, which most philosophers of biology have neglected. Some authors have pointed to methodological limitations with these older studies. However, Grant (Reference Grant1980, 157) clarified that, relatively speaking, these limitations do not vitiate the evidence against gene flow's causal powers, since the same limitations constrain evidence for those powers. More recently, Neigel's (Reference Neigel1997) discussion of gene flow assay methods explained that from the 1960s through to about Reference Neigel1997, virtually all quantitative studies of gene flow employed imperfect, though nonetheless illuminating allozyme methods. Throughout this period, some advocates of The View (e.g., Ghiselin Reference Ghiselin1997, 102) presumed that, at the very least, gene flow is extensive and unifying within sexual marine species that appear to distribute widely via, for example, planktonic larval dispersal. However, significant improvements in methodology since 1997 have bolstered the case against The View, and, ironically, this has been especially true of sexual marine species (e.g., Hellberg et al. Reference Hellberg, Burton, Neigel and Palumbi2002; Bilodeau et al. Reference Bilodeau, Felder and Neigel2005). Reporting on these recent studies, in addition to pre-1997 ones, will prove especially fruitful because to my knowledge they have not been explicitly discussed in connection with the nature of species cohesion.
With the relevant background before us, let us turn to see how gene flow is unnecessary for species cohesion.
4. Gene Flow Unnecessary.
Many sexual animal species consist of populations that seldom if ever exchange genes, but which remain undifferentiated and cohesive nonetheless (Ehrlich and Raven Reference Ehrlich and Raven1969). This is even true of aerial species that are often presumed able to overcome geographic separation. Colonies of the butterfly Euphydryas editha, for example, were found scattered through California with distances of up to 200 km separating them, and yet gene flow between colonies was nearly zero when gaps between them measured as little as 100 m (Ehrlich Reference Ehrlich1965, 327). Yet high levels of evolutionary similarity persist across populations of the species. Thus, “there seems no possibility that gene flow ‘holds together’ its widely scattered population” (Ehrlich and Raven Reference Ehrlich and Raven1969, 1229). Studies of prairie dogs (Chesser Reference Chesser1983), lizards, newts, and numerous bird species (Ehrlich and Raven Reference Ehrlich and Raven1969, 1228) also show that gene flow is circumscribed within populations that no significant geographic barriers seem to divide (1228). Mating naturally occurs in pockets, yet evolutionary similarity persists across these.
Even when ‘travelers’ transgress pocket boundaries, or overcome actual significant geographic separation, they often do not mate with any of their hosts, and when they do manage to mate, they often do not successfully produce offspring. This is evidenced by studies of Mus musculus individuals wandering between granary populations (Ehrlich and Raven Reference Ehrlich and Raven1969, 1229), and by studies of emigrating members of Euphydryas editha (Labine Reference Labine1966, 580). Moreover, when gene flow happens to connect populations, often no novel genes leave lasting genotypic footprints in the population and in such cases preceding gene flow seems insignificant for species cohesion.
Moving to sexually reproducing plants, there is even greater evidence of gene flow being unnecessary for species cohesion. Typically, either wind or insect pollination facilitates sexual reproduction in plants. One might assume that wind facilitates reproduction over vast distances, “but this assumption is not borne out by the available data” (1229). For example, outcrossing in Zea mays (corn) is only 1% at distances greater than 18 m, and in Beta vulgaris (beets) is just 0.3% at distances beyond 200 m; likewise among Coulter pines, successful dispersal does not reach far beyond 10 m (Ehrlich and Raven Reference Ehrlich and Raven1969, 1229). Consequently, Futuyma (Reference Futuyma1998, 317) has summarized that “a large number of crop species have shown that fields separated by a kilometer or more are effectively isolated in most cases.”
Insect pollinated interbreeding fairs no better. In numerous studies of plants, “there is considerable evidence that distances of from 50 feet … to a few miles … may effectively isolate populations, and there is no evidence of longer-range gene flow” (Ehrlich and Raven Reference Ehrlich and Raven1969, 1229). In these studies, high levels of evolutionary similarity persist across populations separated by thousands of kilometers. Based on the illumination of pervasive geographic separation alone, Ehrlich and Raven conclude that in “the vast majority” of species, factors other than gene flow, such as natural selection and developmental homeostasis, unify species (1229). Other investigators corroborated this thesis shortly after its publication (e.g., Endler Reference Endler1973; Lande Reference Lande1980; Grant Reference Grant1980). Natural selection has significant unifying effect within species during, for example, episodes of directional selection, where population level frequencies of certain traits increase and result in higher levels of evolutionary similarity among conspecifics (Morjan and Rieseberg Reference Morjan and Rieseberg2004). Developmental homeostasis can help maintain species cohesion during, for example, potential episodes of divergent selection, when intimate ontogenetic connections between parts of commonly had developmental systems help population level frequencies of these systems to survive evolutionary pressures (Eldredge and Gould Reference Eldredge, Gould and M Schopf1972).
The point of philosophical interest to draw from the above studies is that, contrary to much writing on species in philosophy of biology, gene flow seems unnecessary for the generation of species cohesion in most species; that is, most species comprise populations that are geographically separated in ways that preclude gene flow occurring at all or in any substantial way, and yet those populations continue to constitute evolutionarily cohesive species. The data exhibit the mundane though overlooked point that conspicuous physical barriers often obstruct gene flow that could generate species cohesion. But surprisingly, the data suggest gene flow even fails in the absence of conspicuous physical obstacles. Remarkably short distances in themselves are barriers to gene flow in many species. Thus, given the widely scattered nature of most species, the gene flow required for evolutionary similarity and species cohesion often does not exist. Yet separation does not preclude populations from cohering in the sense that biologists imply when referring to species cohesion.
More recent studies add sophistication to the claim that gene flow is unnecessary for species cohesion. They do so in two ways. First, they add methodological sophistication. For instance, methods utilizing mitochondrial DNA sequences and microsatellite length polymorphism make results similar to those reported above more compelling (e.g., see Hellberg et al. Reference Hellberg, Burton, Neigel and Palumbi2002). But second, these recent studies add explanatory sophistication to the not-necessary claim. They suggest, for instance, that ecological complexities of population structure and dynamics help explain the lack of gene flow in situations where more simplistic ecological presumptions would have motivated the mistaken assumption that rates of gene flow were high.
Bilodeau et al. (Reference Bilodeau, Felder and Neigel2005) invoke such ecological explanations. Their study suggests planktonic larval populations are not as ‘genetically open’ as their spatial proximity implies (151). Analyses indicated, “lack of pronounced genetic differentiation among populations is due to large effective population sizes (reduced genetic drift) rather than high rates of gene flow” (161). This appeal to population structure, rather than gene flow, also fits with growing data on the dynamics of larval transport mechanisms, such that any degree of population homogenization “cannot be simply equated with high rates of gene flow” (161).
Bringing these sophisticated results and explanations into the context of species cohesion, it seems that complexities of populations that we are just beginning to appreciate indicate again that gene flow is unnecessary for species cohesion. Recent studies show that not even modest spatial gaps are necessary to block gene flow; ecological dynamics can ensure there is little gene flow even within contiguous populations. This has motivated collaborations of ecologists and population geneticists, which in turn has revealed that many populations of fish and marine invertebrates seem kept together by factors other than gene flow in “the Atlantic (Pogson et al. 2001), the Mediterranean (Borsa et al. 1997), deep sea (Vrijenhoek 1997), and the tropical Pacific (Palumbi et al. 1997)” (Hellberg et al. Reference Hellberg, Burton, Neigel and Palumbi2002, 282; see source for citations within the quotation).
Summing this section, there are a range of scenarios in which gene flow is not present or significant between populations, but in which those populations instantiate species cohesion. In a great many species where we once thought gene flow was generating species cohesion, gene flow is not the primary factor. Now let me turn to show that in addition to being unnecessary for species cohesion, gene flow is insufficient as well.
5. Gene Flow Insufficient.
There are two senses in which data suggest gene flow is insufficient for species cohesion. There are cases in which gene flow is insufficient to bring distinct populations into a cohesive unit, i.e., ‘generate new cohesion’. And there are cases in which gene flow is insufficient to ‘maintain old cohesion’. Take these in turn.
Templeton's (Reference Templeton, Otte and Endler1989) work shows even high rates of gene flow between populations can fail to bring populations into a cohesive whole. This is clearest in the case of syngameons, which are collections of what most biologists would consider to be populations of distinct species. Despite being of different species, however, populations in a syngameon collective frequently overcome pre-zygotic reproductive barriers. Thus, there is gene flow between distinct species in the syngameon, and yet this is insufficient, even over significant periods of ‘evolutionary time’, to unify the corresponding species, populations, and organisms into one unit that displays a single instance of species cohesion. The distinct but interbreeding populations retain their own instances of species cohesion in virtue of factors such as microclimatic selection regimes that are unique to each of them. Templeton (10–11) puts it thus:
The species within a syngameon are often real units in terms of morphology, ecology, genetics, and evolution. For example, the fossil record indicates that balsam poplars and cottonwoods … have been distinct for at least 12 million years and have generated hybrids throughout this period (Eckenwalder Reference Eckenwalder1984). Even though the hybrids are widespread, fertile, and ancient, these tree species have and are maintaining genetic, phenotypic, and ecological cohesion within and distinction between and have maintained themselves as distinct evolutionary lineages for at least 12 million years (Eckenwalder Reference Eckenwalder1984) … [C]ottonwoods and poplars are real biological units that should not be ignored.
Moreover, the ability to remain distinct in the face of gene flow is not unique to plant species, as many zoologists once believed. Recombinant DNA sequencing techniques show that syngameons are common in all four major mammalian groups and even within Drosophila (Templeton Reference Templeton, Otte and Endler1989, 11).
Turning to cases where gene flow fails to ‘maintain old cohesion’, authors have suggested numerous mathematical models of speciation that suggest selection can overwhelm high rates of gene flow and cause a population to diverge. Such models were once widely thought interesting but seldom instantiated in nature; however, increasingly sophisticated models alleviate such worries. Models of clinal speciation, for example (see Baker Reference Baker2005, 317ff.), show that a population can diverge when there is “a steep environmental gradient across a series of semi-isolated populations, such that selective pressures at one end differ significantly from those at the other end” (317). Gene flow is insufficient to keep the whole population together, and, at the same time, sufficiently distinct selective regimes ensure that each daughter population displays its own distinct cohesion. New models of ecological speciation suggest the same conclusion. Traditional standards of ‘single-locus models’ made it difficult to show how genetic divergence would be initiated during clinal or ecological speciation. But with the increasing suspicion that traditional standards do not respect the complications of nature, clinal and ecological models now seem more compelling. As Baker puts it,
divergent habitat preferences, low hybrid fitness, modifier genes, and other specific genetic and population structures are each unlikely either to emerge in a population or to produce reproductive isolation [but] the likelihood that some combination will do so is much higher. … (Baker Reference Baker2005, 319)
Moreover, studies now document speciation events of these kinds in insects (Bush Reference Bush1994), indigo birds (Sorenson et al. Reference Sorenson, Sefc and Payne2003), a variety of fish (van Alphen et al. Reference van Alphen, Seehausen, Galis, Dieckmann, Doebeli, Metz and Tautz2004) and palms (Savolainen et al. Reference Savolainen, Anstett, Lexer, Hutton, Clarkson, Norup, Powell, Springate, Salamin and Baker2006).
The above-mentioned recent studies of gene flow within planktonic larvae populations also strengthen the empirical case against gene flow's sufficiency for species cohesion. I mentioned that these studies reveal little gene flow between populations; however, within each population, where genes were flowing from parents to offspring, there were sometimes surprising levels of genetic differentiation (Bilodeau et al. Reference Bilodeau, Felder and Neigel2005). For investigators, ecological complexity was again explanatory. For example, they appealed to different kinds of subpopulations that populations comprise. Some of these are genetically differentiated source subpopulations, which contribute organisms to larger sink subpopulations. Because the source subpopulations are genetically differentiated, the sink subpopulations to which they contribute can “themselves … become genetically differentiated” (161). As a result, throughout the population as a whole, the surprising level of genetic differentiation found could be maintained in the face of high levels of gene flow. Bilodeau and colleagues suggest this as an explanation of their data and in doing so they question the common assumption that “any degree of genetic differentiation between marine populations can be interpreted as evidence for restricted gene flow” (161).
The important point to draw from this section is that measures of differentiation in and between populations suggest that high rates of gene flow sometimes fail to generate or maintain the high levels of evolutionary similarity sufficient for species cohesion. Populations can diverge, or remain divergent, despite such flow.
With the empirical argument against The View before us, let me briefly discuss its implications.
6. Implications.
The above argument implies that the question, “What generates high levels of evolutionary similarity among conspecifics and, thereby, generates species cohesion?” is largely an empirical one, the answer to which will depend on the case in question. And we saw that ‘gene flow’ seems not the whole, and sometimes not even a significant part, of the empirical answer in a striking range of cases. Or as others have put it, ‘many’ (Morjan and Rieseberg Reference Morjan and Rieseberg2004, 1341; Ehrlich and Raven Reference Ehrlich and Raven1969, 1229) and perhaps even ‘most’ (Ehrlich and Raven Reference Ehrlich and Raven1969, 1231) cases of species cohesion seem to owe crucially to factors other than or additional to gene flow. So not only are such cases too numerous and varied to be special, but they also suggest that alternative factors to gene flow indeed have wide-spread significance for species cohesion. This rejects The View, as articulated in Section 2. Generally privileging gene flow unjustifiably denies adequate empirical and conceptual attention to other potential and known factors of species cohesion, and thereby obstructs achievement of a more complete understanding of species cohesion.
Biologists convinced of The View's inadequacies have offered related, substantial prescriptions. For example, realizing that colleagues have underestimated cohesion-generating effects of natural selection, Hellberg et al. (Reference Hellberg, Burton, Neigel and Palumbi2002, 273) claim, “Future genetic surveys should include more detailed spatial and temporal sampling and employ analyses of DNA sequence data that can reveal the signatures of natural selection and historical changes.” Morjan and Rieseberg (Reference Morjan and Rieseberg2004) find reasons for thinking that effects of interactions between selection and gene flow have been significantly underestimated and require further study.
Philosophers of biology have not considered the philosophical aspects of such remarks. For instance, although some have been critical enough of The View to endorse pluralistic views of species cohesion, only a few (e.g., Wilson Reference Wilson2005) have realized that affective interactions between different factors of species cohesion suggest that more integrative accounts of species cohesion are in order. Such considerations could surely influence broader views and debates. Many definitions of ‘species’ have depended on accounts of species cohesion, and the way one opts in more general debates between pluralistic and integrative views of scientific kinds can crucially influence how one thinks science should be conducted, funded and governed. Rather than discuss implications for these broader views here, however, I want, in closing, to point to a possible implication of the above argument that requires discussion before implications for broader views are assessed.
The empirical problems raised above may suggest that authors have incorrectly conceptualized the notions of species cohesion and gene flow. Indeed, it may be that many authors have missed the empirical problems just because they have operated with notions of species cohesion and gene flow that are conceptually inadequate for empirical complexities at hand. To give this suggestion prima facie plausibility, consider that both notions are clearly metaphors, and yet their status as such has received no discussion. Cohesion, on the one hand, is literally the state of being unified or bonded; yet species are collections of discrete organisms that only cohere in a non-literal, materially discontinuous sense. That is, species are not cohesive in and of themselves, but only metaphorically, with respect to evolutionary pressures. Gene flow, on the other hand, conjures images of strips of DNA traveling through multiple organisms, across multiple generations; yet no token strip travels as such, since each is at best represented in copies across multiple generations. These metaphors may be necessary, and explanatorily helpful. However, we must appreciate their limits. I suspect that further probing of them will reveal there is no sense in which gene flow materially integrates species. As a result, the corresponding cohesion is more like uniformity than integration. Authors have briefly hinted at such a distinction (e.g., Ereshefsky Reference Ereshefsky1988). If one can develop this distinction and show that it marks a distinction between kinds (rather than just degrees) of cohesion (see Barker Reference Barker2005), then standard arguments for The View are likely to equivocate on ‘species cohesion’. Understanding these conceptual problems may help further illuminate the empirical problems, and pursuing them is likely a prerequisite for assessing exactly how problems for The View vitiate other views that depend upon it.