


INTRODUCTION
Oysters have contributed to the ecology and geomorphology of temperate estuarine habitats for at least 200 million years (Stenzel, Reference Stenzel and Moore1971). The eastern oyster Crassostrea virginica (Gmelin 1791) occupies coastal habitats in the western Atlantic from Canada to Argentina (Carriker & Gaffney, Reference Carriker, Gaffney, Kennedy, Newell and Eble1996). These bivalves have been considered keystone species because of their roles as ecological and habitat engineers through benthic pelagic coupling (e.g. Dame et al., Reference Dame, Zingmark and Haskin1984; Newell, Reference Newell, Lynch and Mihursky1988; Ulanowicz & Tuttle, Reference Ulanowicz and Tuttle1992; Kennedy, Reference Kennedy1996) and construction of biogenic hard substrate habitat through recruitment and shell growth (e.g. Bahr & Lanier, Reference Bahr and Lanier1981; Powell et al., Reference Powell, Kraeuter and Ashton-Alcox2006). Observed oyster population dynamics result from the interaction of recruitment, individual growth, reproduction and mortality. Reproduction sets the stage for recruitment. Fecundity scales linearly with biomass (Bayne et al., 1983) and non-linearly with length (Cox & Mann, Reference Cox and Mann1992; Thompson et al., Reference Thompson, Newell, Kennedy, Mann, Kennedy, Newell and Eble1996). Mortality sets the boundaries for functional reproductive populations because it constrains life expectancy and selects for adaptations in reproductive and life history strategy.
Oysters in the genus Crassostrea are sequential protandrous hermaphrodites (Andrews, Reference Andrews, Giese and Pearse1979; Kennedy, Reference Kennedy1983; Guo et al., Reference Guo, Hedgecock, Herhberger, Cooper and Allen1998). Smaller individuals are generally male with maturity at approximately 35 mm shell length and ages of less than 1 year (Burkenroad, Reference Burkenroad1931; Coe, Reference Coe1936; Dinamani, Reference Dinamani1974; Kennedy, Reference Kennedy1983; O'Beirn et al., Reference O'Beirn, Walker and Jansen1998). The proportion of females in a population increases with increasing size and age (Dinamani, Reference Dinamani1974; Andrews, Reference Andrews, Giese and Pearse1979; Kennedy, Reference Kennedy1983; Heffernan et al., Reference Heffernan, Walker and Carr1989). The timing of the transition from male to female is selected to optimize the reproductive potential of both sexes (Morbey & Abrams, 2004). This life history strategy evolved in concert with oyster life spans in excess of 6 years (Comfort, Reference Comfort1957) and probably on the order of 10–20 years (Powell & Cummins, Reference Powell and Cummins1985; Kirby, Reference Kirby2000).
Sex in Crassostrea is determined by a two allele system (Guo et al., Reference Guo, Hedgecock, Herhberger, Cooper and Allen1998) in which the dominant allele is male (M) and the recessive allele is protandric (F). The presence of permanent males (MF) within a population acts to stabilize the sex-ratio in long-lived animals (Powell et al., Reference Powell, Klinck and Hofmann2010) in that these individuals will constrain the observed sex-ratio to 3:1 or 75% female. There is evidence that natural habitat factors may modulate sex-ratios with an increase in functional males observed at higher densities (Buroker, Reference Buroker1983; Kennedy, Reference Kennedy1983) and under stressful environmental conditions (Kennedy, Reference Kennedy1983).
Historically, Chesapeake Bay oyster (C. virginica) populations occupied large portions of the mesohaline tributaries and their reefs extended from the substrate through the water column and were exposed intertidally (Hargis, Reference Hargis, Luckenbach, Mann and Wesson1999; Woods et al., Reference Woods, Hargis, Hershner and Mason2005). Modern Virginia oyster populations are reduced from historic levels in both numbers (Rothschild et al., Reference Rothschild, Ault and Heral1994) and spatial extent (Haven et al., Reference Haven, Hargis and Kendall1978; Haven & Whitcomb, Reference Haven and Whitcomb1986). Natural mortality from predation is compounded by fishing and disease mortality from Dermo (Perkinsus marinus) and MSX (Haplosporidium nelsoni). Disease has been an important factor influencing Virginia oyster populations since the introduction of MSX in 1959 (Andrews & Wood, Reference Andrews and Wood1967) and the intensification of Dermo with the drought conditions of the 1980s (Andrews, Reference Andrews1996; Burreson & Ragone Calvo, Reference Burreson and Ragone Calvo1996). Mortality from both fishing and disease target older, larger oysters and potentially have a disproportionate impact on females effectively imposing size and age specific cropping. Fishing pressure may be managed, but disease mortality is constrained only by ambient conditions of temperature and salinity with reduced levels of both acting to reduce mortality (Burreson & Ragone Calvo, Reference Burreson and Ragone Calvo1996; Cook et al., Reference Cook, Folli, Klinck, Ford and Miller1998; Soniat et al., Reference Soniat, Hofmann, Klinck and Powell2009).
Size-specific cropping selects for slower growing, smaller and younger individuals that reach maturity earlier (Law & Grey, Reference Law and Grey1989; Buxton, Reference Buxton1993; Rochet, Reference Rochet1998; Walsh et al., Reference Walsh, Munch, Chiba and Conover2006). While these traits may be adaptive in high mortality situations, historically oysters used an opposite approach where fast growth to indeterminate body size decreased the time to achieve size-related predation refugia while positively affecting fecundity and maintenance of the habitat/shell base required for recruitment and natural self-sustaining populations. Sustained selection for life history traits favoured by size-specific cropping over decadal scales will place populations at a disadvantage if the selective pressures are removed or modulated and the organisms are required to function at the original conditions (Law & Grey, Reference Law and Grey1989; Walsh et al., Reference Walsh, Munch, Chiba and Conover2006).
Oyster life history strategies are presumably optimized for their historical life expectancy of 10–12 years (Powell & Cummins, Reference Powell and Cummins1985) and natural mortality rates. Changes in oyster life expectancy and mortality rates in Virginia (or Chesapeake Bay) have been ongoing since at least 1607 with the arrival of European colonists but have accelerated since the 1980s due to the combination of oyster diseases, harvest activity and environmental conditions. Current Virginia oyster populations have truncated demographics whereby older individuals are rare and suffer under annual mortality rates (natural, disease and fishing mortality combined) in excess of 60% (Mann et al., Reference Mann, Southworth, Harding and Wesson2009a; Harding et al., Reference Harding, Mann, Southworth and Wesson2010; Southworth et al., Reference Southworth, Harding, Mann and Wesson2010). Since protandry is predicated on optimizing female lifetime reproductive capacity (Powell et al., Reference Powell, Morson, Ashton-Alcox and Kim2012) the observed reduction in Virginia oyster life expectancy likely has consequences for the timing of the protandric shift and associated sex-ratios. Thus, sex-ratios from oyster populations representing a range of Virginia oyster habitats provide information about population dynamics that is fundamental to understanding population function since the disease epizootics of the late 1980s. We describe oyster population sex-ratios in three Virginia tributaries with regard to length and age during 2008. The resulting data are incorporated into sex–age and sex–length keys that are used with stock assessment data to describe the proportion of landings that are female and population dynamics over multiple years (2006–2009).
MATERIALS AND METHODS
A size-range of 100 oysters was collected from each of twelve natural bars in the James, Rappahannock, and Great Wicomico Rivers (Figure 1; Table 1) once per month in June, July and August 2008 when water temperatures exceeded 18–20°C and visual observations of oyster gonads indicated that they were ready to spawn. Collections included the entire available shell length range for each bar. The bars were chosen to span a latitudinal gradient and include sites for which long-term datasets on oysters, water temperature and salinity are available. All twelve sites are included in the autumn oyster surveys conducted by the Virginia Institute of Marine Science Molluscan Ecology Program in collaboration with the Virginia Marine Resources Commission (e.g. Mann et al., Reference Mann, Southworth, Harding and Wesson2009a; Southworth et al., Reference Southworth, Harding and Mann2009, Reference Southworth, Harding, Mann and Wesson2010).
Map of the twelve oyster bars in the James, Rappahannock, and Great Wicomico Rivers sampled (Table 1) including: Deep Water Shoal (A); Middle Horsehead (B); Point of Shoals (C); V Rock (D); Wreck Shoal (E); Brown Shoal (F); Thomas Rock (G); Nansemond Ridge (H); Drumming Ground (I); Parrot Rock (J); Broad Creek (K); and Shell Bar (L). Hydrographic monitoring stations were located at Gloucester Point (M), Middle Ground (N), Drumming Ground, Broad Creek, and Shell Bar.

Summary of oyster bars and age–length relationships with group classifications from the James, Rappahannock (Rap) and Great Wicomico (GW) Rivers sampled during 2008. Bar abbreviations correspond to labels on Figure 1. Groups 1–5 reflect river specific groups with age–length relationships that are statistically distinct from each other (analysis of covariance, P < 0.05). n is the number of oysters from a bar that contributed to the linear regression (age = m * (SL) + b) of shell length (SL, mm) with age (yr) where m is the slope and b is the y-intercept. Coefficients of determination (R2) are provided for the bar-specific length–age regressions. The regression for Wreck Shoal, Thomas Rock, Brown Shoal, and Nansemond Ridge is from Harding et al. (Reference Harding, Mann and Southworth2008).

Water temperatures for Deep Water Shoal (Figure 1; Table 1) were described using data from a York River (37°14′47″N 76°30′23″W) monitoring station as a surrogate (Mann & Evans, Reference Mann and Evans1998; Mann et al., Reference Mann, Southworth, Harding and Wesson2009a). Monthly average salinities for Deep Water Shoal were calculated from daily US Geological Survey (USGS) gauge data (2005–2008) at Richmond following Mann & Evans (Reference Mann and Evans1998) with the correction identified by Mann et al. Reference Mann, Southworth, Harding and Wesson(2009a).
Water temperatures measured near Nansemond Ridge (36°56′42.4″N 76°23′29.6″W) from March 2007 through to 2008 were used to estimate water temperatures for Wreck Shoal, Thomas Rock, Brown Shoal and Nansemond Ridge (Figure 1; Table 1). Salinities for these four bars were calculated by combining salinities estimated for Wreck Shoal from USGS daily discharge data (per Mann & Evans, Reference Mann and Evans1998) with salinities measured near Nansemond Ridge (36°56′42.4″N 76°23′29.6″W).
Water temperature and salinity were measured near the survey bars in the Rappahannock and Great Wicomico Rivers from 2005 through to 2008. Data from hydrographic monitoring stations near Drumming Ground (37°34′39″N 76°19′09″W), Broad Creek (37°39′10″N 75°27′40″W), and Shell Bar (37°49′46″N 76°19′08″W) were used to calculate average monthly water temperatures and salinities during 2005–2008 to describe the general range of environmental conditions for the Rappahannock and Great Wicomico survey bars (Figure 1; Table 1).
Oysters were measured (shell length (SL) the longest distance from the hinge to the growth edge, mm) in the laboratory and opened while live. Once opened, oysters were classified as female, male, hermaphrodite, or indeterminate through examination of gonad material under a compound microscope at 100–400× magnification. Only eggs were observed in female gonads while male gonads had only sperm. Hermaphrodites had both eggs and sperm visible in their gonads. Indeterminate oysters did not have enough visible gonad to determine their sex. Multiple gonad samples were removed from all hermaphrodites and every fifth pure individual to verify the initial sex determination.
Sex-ratios, described as the fraction of females (Females/[Females + Males]), were obtained by calculating a sex-at-length key for each bar. Within a bar, data were pooled across months to ensure that each site was represented by 250–300 individuals with at least 5 individuals per 10-mm SL class throughout the available size-range. Monthly collections alone did not yield suitable n values for analyses with month as a factor. Shell lengths were used to characterize the population demographic for each bar.
Biomass (dry tissue weight (DTW g)) was determined for a size-range of oysters from each bar. Oysters were measured (SL, mm) and then tissue was separated from the shell and dried to constant weight (80°C for 72 hours) in individually labelled and weighed pans. The relationship between SL (g) and biomass DTW, g was described for each bar with a power regression (DTW = a * SLb); where a and b are regression coefficients. Biomass data were combined with length and sex data to calculate a sex–biomass key.
Individual oyster SL measurements (mm) from autumn surveys on each bar in 2006, 2007 and 2008 were grouped into 2-mm bins and used to describe bar-specific age-at-length relationships. Cohort analyses were applied to each bar-specific data set using the methods described by Bhattacharya (Reference Bhattacharya1967) previously applied to James River (Mann et al., Reference Mann, Southworth, Harding and Wesson2009a) and Great Wicomico River (Southworth et al., Reference Southworth, Harding, Mann and Wesson2010) oyster populations. Shell lengths were converted to ages for each bar. Age–length relationships were compared among bars using analyses of covariance (ANCOVAs). The alpha value for all statistical tests was set at 0.05 a priori. Bars within an estuary (James, Rappahannock or Great Wicomico) with similar age–length relationships were then grouped for all subsequent analyses (Table 1). Sex-ratio data were recast on the basis of age using 1-year bins resulting in a sex-at-age key for the groups of interest.
Bar-specific length data from oyster stock assessment surveys in autumn 2006, 2007 2008 and 2009 were used in concert with sex–length, sex–age, and sex–biomass keys developed above to describe population (standing stock, number bar−1) sex-ratio dynamics with regard to length, age, and biomass for each year. Stock assessment data for each bar include individual measurements of all live oysters encountered on a m−2 basis (methods are discussed in Mann et al., Reference Mann, Southworth, Harding and Wesson2009a; Harding et al., Reference Harding, Mann, Southworth and Wesson2010; Southworth et al., Reference Southworth, Harding, Mann and Wesson2010). These data were incorporated into weight group sex-ratios by observed bar and year-specific standing stock demographics using 10-mm SL bins.
Statistical analyses followed Powell et al. (Reference Powell, Morson, Ashton-Alcox and Kim2012). Comparisons of sex-ratios were made with binomial statistics (Conover, Reference Conover1980). Although many more individuals were measured to establish population demographics than were examined to determine sex-ratio, the n values of the sex-ratio dataset were maintained for analyses by proportionately reducing the population data to a total number of oysters equal to the number used to determine sex-ratio. This normalization procedure corrected each bar-specific data set resulting in conservative population descriptions.
The relationship between the fraction female by group was described with a three parameter Gompertz model where:
 $$\hbox{Fraction female} = Alpha\,{\ast}\, e^{Beta^{\ast} e^{Gamma^{\ast} Length\lpar mm\rpar }}$$
Gompertz curves were compared between groups using randomization tests (Noreen, Reference Noreen1989) per Powell et al. (Reference Powell, Morson, Ashton-Alcox and Kim2012).
RESULTS
The three rivers included in the study had average monthly water temperatures within 1–2°C of each other (Supplementary Material 1). Seasonal minima (~5–6°C) were observed in January or February with seasonal maxima observed in August (~28°C). There was a stronger salinity gradient observed within the James River between Deep Water Shoal (Group 1, upriver) and Wreck Shoal, Thomas Rock, Brown Shoal and Nansemond Ridge (Group 3, downriver) than between Rappahannock River bars (Broad Creek, Parrot Rock and Drumming Ground: Group 4) and Shell Bar in the Great Wicomico River (Group 5). Salinities in the James River were lowest in April (Group 1 = 4.15 and Group 3 = 10.92) during the spring rainy season but still within the range of oyster salinity tolerance (Gunter, Reference Gunter1950; Butler, Reference Butler1952; Galtsoff, Reference Galtsoff1964). The salinities observed in the Rappahannock and Great Wicomico Rivers year round as well as in the James River from June through October represent the intermediate salinity range suggested as physiologically optimal (R. Newell in Shumway, Reference Shumway, Kennedy, Newell and Eble1996).
Oysters from all bars were primarily within the 30–120 mm SL range with the outgroup of 120+ mm SL oysters representing 1.7% of the 3597 oysters examined. The majority (97.4%) of these oysters were in the 40 to 90 mm SL range and Age 1 and Age 2 year-classes regardless of bar or month (Supplementary Material 2). Oysters Age 4 and older composed 2.6% of all oysters examined and were not observed on Point of Shoal, V Rock or Shell Bar (Supplementary Material 2). An insufficient number of oysters were represented in the smaller (<30 mm SL or Age 0; Supplementary Material 2) and larger/older classes (>100 mm SL or Age 4 and older; Supplementary Material 2) for both length and age distributions within a particular bar and month for statistical analysis. Thus, bar-specific data from June, July and August 2008 were pooled across months within a length or age-class to increase the number of oysters for analyses (Supplementary Material 3). Subsequently, within the 30-to-100-mm length and 1-to-4-yr age-classes, sex was determined for at least 20 individuals sexed within each class. Shell length bins <30 mm were excluded from all analyses due to insufficient sample size (Supplementary Material 3).
The fraction of oysters examined that were female, irrespective of hermaphrodites or indeterminate individuals, increased within increasing size and age (Supplementary Material 2). The fraction female across all bars increased from 0.09–0.30 in the 30–39 mm size-class to 0.4–0.88 in the 100–109 mm size-class. Fraction female values of 1 were observed at several bars in the size-classes larger than 100 mm SL although these values result from examination of <10 individuals (Supplementary Material 2). The fraction female in the Age 0 year-class ranged from 0 to 0.36 (Supplementary Material 2). With the exception of Broad Creek, the fraction female in Age 3+ groups was more than 50% (Supplementary Material 2).
Simultaneous hermaphrodites were rarely (16 of 3597 oysters examined or 0.4%) observed at most bars (Supplementary Material 4) in any size or age-class. Hermaphrodites were found exclusively in July and August and most were observed at Thomas Rock in the lower James River in the 50–80 mm length-classes. Simultaneous hermaphrodites were excluded from further analyses because they occurred so infrequently.
Although the sex of most oysters could be determined, a fraction of the population at each bar was usually indeterminate irrespective of size or age-class (Supplementary Material 5). In general, incidence of indeterminate oysters decreased with increasing size and age. Of the 3597 oysters examined, 8% were indeterminate with most (94%) of these occurring in July and August, presumably after oysters had spawned at least once and were in the process of reconditioning. Indeterminate oysters were not included in any further analyses.
Data from the James River bars were pooled on the basis of similarities between linear age–length relationships (ANCOVA, P < 0.05) into three groups: Group 1 (Deep Water Shoal), Group 2 (Point of Shoals, V Rock and Middle Horsehead), and Group 3 (Wreck Shoal, Thomas Rock, Brown Shoal and Nansemond Ridge: Table 2). Data from bars within the Rappahannock and Great Wicomico Rivers were combined into river-specific groups (Groups 4 and 5, respectively: Table 2). Sex-at-length keys were applied to each group-specific length–frequency distribution observed during summer 2008 to calculate group-specific population sex-ratios (Figure 2). The sex-ratio would be the same for the entire group if sex-at-age had been used because the same individuals were used to generate the group specific frequency distribution whether by length or age.
The fraction female for the oyster population in each bar group from collections made in June–August 2008 based on length (A) and age (B). Bar-groups within the James River are based on similarities in length–age relationships: Group 1 (Deep Water Shoal); Group 2 (Point of Shoals, V-Rock and Middle Horsehead); and Group 3 (Wreck Shoal, Thomas Rock, Brown Shoal and Nansemond Ridge). Data from bars within the Rappahannock and Great Wicomico Rivers were combined into river-specific groups (Groups 4 and 5, respectively). The fraction female ratios are corrected for the size–frequency upon collection for each individual bed and the bed sample values summed to provide group estimates uncorrected for variation in total oyster abundance between beds. The P values obtained from binomial tests with an expected fraction of 0.5 (a 1:1 female:male ratio) are presented above each bar. Asterisks indicate values that are significantly different from a 1:1 female:male ratio.

The fraction of female oysters by bar group for length (A) and age-classes (B). Groups are identified in Table 1. Column headings are the midpoint of the length or age-classes. ‘nan’ indicates not enough oysters to calculate; * indicates length or age-classes with <10 oysters.

The fraction of females observed within groups across length and age-classes (Table 2) was significantly different from 1:1 only in Groups 1 and 3 (Figure 2). Group 1 had more females than males while Group 3 had more males than females. Binomial tests to evaluate the deviation of the fraction females observed within a group by length and age-classes (Table 3) indicate an intermediate size/age range with approximately equal numbers of males and females bounded by smaller/younger male oysters (Table 4) and larger/older female oysters (Table 5).
Binomial test results examining the divergence of sex-ratios in Table 2 from 1:1 or equal probability of male and female with regard to length (A) and age (B). ‘nan’ indicates not enough oysters in the length or age-class to calculate; ‘ns’ indicates that the binomial test results were not significant at alpha = 0.05.

Binomial test results examining the divergence of sex-ratios in Table 2 from 0% or all male expected for smaller/younger oysters with regard to length (A) and age (B). ‘nan’ indicates not enough oysters in the length or age-class to calculate; ‘ns’ indicates that the binomial test results were not significant at alpha = 0.05.

Binomial test results examining the divergence of sex-ratios in Table 2 from 3:1, the 75% female condition expected for larger/older oysters with regard to length (A) and age (B). ‘nan’ indicates not enough oysters in the length or age-class to calculate; ‘ns’ indicates that the binomial test results were not significant at alpha = 0.05.

The fitted Gompertz models (Figure 3) from the sex–length and sex–age keys show a gradient across groups for the timing of the sex-ratio transition from predominantly males to females. The 1:1 female to male transition occurs at shell lengths of 59, 61, 63, 73 and 81 mm for Groups 4, 1, 5, 2 and 3, respectively (Figure 3A). If oyster size-classes from 30 to 120 mm are considered, Groups 1 and 5 have sex-ratios approaching 100% females with increasing size while Groups 2, 3 and 4 are approximately 70% female. However, the ratios for size-classes >100 mm SL are based on fewer than 10 individuals. If only size-classes with more than 10 oysters are considered (i.e. SL < 100 mm), all groups were 70–80% female (Table 2). The transition from a balanced sex-ratio corresponds to average ages of 1.6, 1.8, 2.1, 2.15 and 2.6 years for Groups 5, 2, 1, 4, and 3, respectively (Figure 3B). Sex-ratios never exceed 80% females regardless of age if only age-classes with more than 10 individuals are considered (Table 2). The oldest Group 2 oysters (4.5 years) were 100% female but there were fewer than 10 individuals examined. Results from randomization tests comparing group-specific Gompertz curves indicate that all curves are significantly different from each other at the 0.05 level.
Sex-at-length (A) and sex-at-age (B) keys for oyster groups from Gompertz curves describing the fraction female by group for length and age. Equation parameters are given in Table 7.

Subsequent population level analyses took into account variations in abundance and demographics between groups by using bar and year-specific stock assessment data collected in November 2006, 2007, 2008 and 2009. Oysters larger than 100 mm SL occurred more frequently in Groups 2 and 3 than other groups but were still relatively rare overall (Figure 4). Strong recruitment was observed during 2008 for Groups 1, 2 and 3 (all James River) but not for Groups 4 and 5.
Population demographics (shell length, mm) from fishery independent stock assessment surveys during November 2006, 2007, 2008 and 2009 for Groups 1 through to 5 (A–E).

The application of the sex–length key to the population survey data from November 2006–2009 showed that the female fraction of the population ranged from 0.34 to 0.55 (Figure 5A). Within groups, relatively few inter-annual variations in the fraction female were observed. That is, sex-ratios by length were stable within groups over multiple years in keeping with the observed demographic trends (Figure 4). By length, the lowest sex-ratios were generally observed in Group 3 with the highest sex-ratios observed in Group 1. These trends are in keeping with the timing of the protandric shift and the earliest maturation in Group 1 with the latest observed in Group 3.
The fraction female for Groups 1 through to 5 by year normalized for the population using survey data from November of each year based on shell length (A) and biomass (B).

Application of the sex–biomass key (Table 6) to the survey data from 2006 through to 2009 reveals low inter-annual variability in sex-ratios within sites and a high proportion of the standing stock as females (0.60–0.80; Figure 5B). Assuming biomass is a representative surrogate for fecundity, this apparent relative stability in sex-ratios within groups over time indicates similar reproductive contributions across years.
Summary of bar-specific shell length–biomass power regression models. n is the number of oysters from a bar that contributed to the power regression (biomass = a[SL]b) of shell length (SL, mm) with biomass (g) where a and b are regression coefficients. Coefficients of determination (R2) are provided for the bar-specific length–age regressions.

Parameters for the Gompertz equation fits for each group describing the relationship between fraction female and length or age. The equation is:
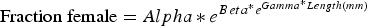 $\hbox{Fraction female} = Alpha\,{\ast}\, e^{Beta^{\ast} e^{Gamma^{\ast} Length\lpar mm\rpar }}$

DISCUSSION
Three of the five bar groups examined displayed balanced (1:1) sex-ratios in keeping with previous observations (Kennedy, Reference Kennedy1983) for subtidal oyster populations in the Maryland waters of the Chesapeake Bay. Two groups within the James River (Group 1 and Group 3) displayed sex-ratios that were skewed toward females and males, respectively. These groups represent outliers relative to the other sites studied. Group 1, Deep Water Shoal, occupies a unique geographical position among all locations examined in that it is the most upriver (lowest salinity) site and is subject to changes in salinity related to seasonal fluctuations in river discharge due to the spring wet season (Supplementary Material 1). While it is subjected to fishing pressure, its location on the salinity gradient may offer the potential for the expulsion or removal of one or both diseases (MSX, Dermo) when spring salinities decline below the salinity tolerance of either (salinity tolerance of 3 for Dermo: Burreson & Ragone Calvo, Reference Burreson and Ragone Calvo1996: salinity tolerance of 10 for MSX: Andrews, Reference Andrews1988; Burreson & Ragone Calvo, Reference Burreson and Ragone Calvo1996). Group 3 is composed of four bars that are traditionally subjected to intense fishing pressure during the winter fishing season, intense disease pressure during summer and autumn because of their location within the James River estuarine salinity gradient (Figure 1; Supplementary Material 1), as well as predation pressure from blue crabs (Callinectes sapidus) and veined rapa whelks (Rapana venosa: Harding & Mann, Reference Harding and Mann1999, Reference Harding and Mann2005). Dynamics observed at Group 3 potentially represent the strongest interaction of disease, predation, and fishing pressure on any of the populations examined.
In general, the larger and older oysters have sex-ratios that were 70–80% female, in keeping with the 3:1 balance predicted by the presence of MF individuals (Guo et al., Reference Guo, Hedgecock, Herhberger, Cooper and Allen1998; Powell et al., Reference Powell, Klinck and Hofmann2010). The largest and oldest oysters were poorly represented in the population. If the upper size/age bins with low sample sizes are considered, Groups 1 and 5, characterized by relatively slow growth rates and truncated population demographics, have sex-ratios >80% at SL > 100 mm. By age, Group 2 has the oldest oysters that reach the largest sizes and corresponding sex-ratios approaching 100% female for the available individuals examined (<10).
Oysters spawn at least twice per year in Virginia (Cox & Mann, Reference Cox and Mann1992; Mann et al., Reference Mann, Rainer and Morales-Alamo1994) and there is evidence that C. virginica begins new gonadal development after the initial spawning (e.g. Hayes & Menzel, Reference Hayes and Menzel1981). Simultaneous hermaphrodites have been suggested as the transition phase from male to female that occurs primarily between spawning events (Coe, Reference Coe1943; Tranter, Reference Tranter1958; Asif, Reference Asif1979; Paniagua-Chavez & Acosta-Ruiz, Reference Paniagua-Chavez and Acosta-Ruiz1995; Perharda et al., Reference Perharda, Mladineo, Bolotin, Kekez and Skaramuca2006). Although hermaphrodites were rarely observed, the timing (July–August), and the SL range (50–80 mm) of these observations lend support to the idea that hermaphroditism is symptomatic of the transition from male to female.
The timing of the protandric switch varies with location, size and age. Groups 1, 4 and 5 undergo the change from male to female at smaller sizes than Groups 2 and 3. All groups except Group 3, transition from 1:1 sex-ratios before they recruit to the fishery at shell lengths larger than 76 mm. Given that the transition from male-dominated to female-dominated sex-ratios does not occur in Group 3 until ~80 mm SL, oysters that are fishery targets have a higher likelihood of being male at Group 3 than elsewhere because oysters may be preferentially removed by the fishery before they transition to female. In general, the Virginia oyster fishery is strongly skewed toward females (Figure 6).
The fraction of market oysters (>75 mm shell length) on the bars examined that were female estimated from 2006, 2007, 2008 and 2009 stock assessment surveys using the sex-at-length key described above and the survey values obtained in November of the respective years.

All populations examined have more than 50% females in age-classes older than Age 2.6 years. With a life-expectancy of 3–4 years, this allows reproduction as a female for potentially 1 but probably no more than 2 reproductive seasons, with the possible exception of Group 1, which experiences the protandric shift at Age 1.6 years. The combination of the timing of the protandric shift with age for these Virginia oyster populations is in stark contrast to the dynamics observed during 2008 in Delaware Bay oysters (Powell et al., Reference Powell, Morson, Ashton-Alcox and Kim2012). With life expectancies of ~10–12 years, the timing of the protandric shift does not occur until Age 3–3.5 years for three out of four populations examined in Delaware Bay with the low mortality beds remaining predominantly male until ~Age 5. Delaware Bay oysters potentially function as females for multiple reproductive seasons at larger shell lengths increasing their lifetime fecundity contributions well above those expected for Virginia oysters.
Oysters naturally occur in aggregated spatial distributions by virtue of both their gregarious settlement behaviour and settlement preference for oyster shell substrate. These behaviours are a fundamental part of a life history strategy that maximizes fertilization efficiency and results in the formation and maintenance of large reef structures. Variance to mean ratios (VMR: Supplementary Material 6) calculated from survey data indicate that Virginia oysters within all groups examined were aggregated spatially (VMR > 1: Krebs, Reference Krebs1989). Groups 1, 2 and 5 had VMR ratios that were higher than Groups 3 and 4 (Supplementary Material 6). At higher densities, sex-ratios tend to be skewed toward males (Burkenroad, Reference Burkenroad1931; Menzel, Reference Menzel1951; Kennedy, Reference Kennedy1983). Burkenroad (Reference Burkenroad1931) and Buroker (Reference Buroker1983) observed more males in clusters of oysters and found that single oysters were usually female. The groups with the highest densities in autumn 2007 (Groups 2 and 5; Supplementary Material 6) had the earliest transition from male to female and sex- ratios that were ~1:1 in summer 2008. Among the groups examined, Group 3 had the lowest densities in autumn 2007 (Supplementary Material 6), a sex-ratio skewed toward males, and the protandric switch occurred at larger sizes and older ages than for any other group during summer 2008.
Size and age specific exploitation of populations applies directional selection pressure that favours slow growth, small size, and earlier maturation (Law & Grey, Reference Law and Grey1989; Buxton, Reference Buxton1993; Barot et al., Reference Barot, Heino, O'Brien and Dieckmann2004; Olsen et al., Reference Olsen, Helme, Lilly, Morgan, Brattey, Ernande and Dieckmann2004; Walsh et al., Reference Walsh, Munch, Chiba and Conover2006). Virginia oysters have been intensively fished for the last 400 years, with records of depleted oyster grounds dating to at least the mid-1830s (Rountree et al., Reference Rountree, Clark and Mountford2007; p 140: Nansemond River bars). With the development of organized post-colonization fishing activity, advances in technology have sequentially increased the fishing pressure on Virginia oyster populations (Moore, Reference Moore1897; Haven et al., Reference Haven, Hargis and Kendall1978). Since the introduction of MSX in the late 1950s (Andrews & Wood, Reference Andrews and Wood1967; Andrews, Reference Andrews1968), disease pressure from MSX has compounded the existing pressure from Dermo (Andrews, Reference Andrews1996) exerting age-related mortality on oysters independent of fishery activity and effectively increasing selection pressure on all age-classes beyond the young-of-the-year. In 2008, MSX was absent from Group 1 and Group 2 and present in 8–20% of oysters examined from Group 3 (Carnegie & Burreson, Reference Carnegie and Burreson2009). In contrast, Dermo was present in Groups 1, 2 and 3 with late summer and autumn prevalence values ranging from 36 to 100% (Carnegie & Burreson, Reference Carnegie and Burreson2009). While MSX data are not available for Groups 4 or 5 in 2008, Dermo was observed in Groups 4 and 5 during autumn surveys with high prevalences (72–96%: Carnegie & Burreson, Reference Carnegie and Burreson2009). Thus, Dermo was likely the primary source of non-fishing mortality on oysters from all groups in 2008.
The cumulative combination of centuries of fishing pressure with disease history since the 1980s suggests that current Virginia oyster populations are subject to a set of selection pressures that have not previously been experienced and for which their compensatory ability is still developing. These modern pressures have resulted in a maximum life expectancy of ~5 years with the majority of individuals Age 3 or less for the Virginia oyster populations that have been described to date (Harding et al., Reference Harding, Mann and Southworth2008, Reference Harding, Mann, Southworth and Wesson2010; Mann et al., Reference Mann, Southworth, Harding and Wesson2009a; Southworth et al., Reference Southworth, Harding, Mann and Wesson2010; present study). The corresponding age at which 50% of the population is mature females ranges from 1.6 to 2.6 years. No previous size or age-specific sex-ratio data-sets for these Virginia oyster populations can be used to place the current size/age for the protandric shift in historic context.
Crassostrine oysters were historically long-lived (10–20 years: Powell & Cummins, Reference Powell and Cummins1985; Kirby, Reference Kirby2000) and their life history strategies presumably were optimized for this life expectancy range. The protandrous life history strategy whereby younger individuals are male and older individuals are female is predicated on optimizing female lifetime reproductive capacity (Powell et al., Reference Powell, Morson, Ashton-Alcox and Kim2012) and related to male life expectancy (Morbrey & Abrams, Reference Morbrey and Abrams2004). Mortality rates in excess of 60% have been described for Age 2+ oysters on natural oyster bars in the James (Mann et al., Reference Mann, Southworth, Harding and Wesson2009a), Great Wicomico (Southworth et al., Reference Southworth, Harding, Mann and Wesson2010) and Piankatank Rivers (Harding et al., Reference Harding, Mann, Southworth and Wesson2010) during 2000–2008. These high mortality rates exert selection pressure for traits that were not previously favoured. Even if harvest pressure were reduced or removed, the unpredictable nature of the diseases from year to year, in concert with variable environmental conditions, would force the oysters to cope with selection pressures at time scales shorter than life expectancy before European colonization, intensive harvest during the 1800s, the introduction of MSX (1959) and amplification and spread of Dermo by drought conditions (late 1980s).
The truncation of Virginia oyster population demographics due to the interaction between age-specific harvest and disease pressures is likely to continue for the foreseeable future resulting in oysters with essentially an opportunistic life history strategy favouring earlier maturation at smaller shell length. Given that fecundity in oysters scales non-linearly with shell length, the current selection trend imposed by age and size specific cropping may reduce life-time fecundity estimates and the resulting larval supply for continued propagation of wild oyster populations. Beyond actual mortality, documented disease effects include reductions in biomass and fecundity (Barber et al., Reference Barber, Ford and Haskin1988; Kennedy et al., Reference Kennedy, Newell, Krantz and Otto1995; Paynter, Reference Paynter1996) further reducing ambient propagule pressure and larval supply.
Continued truncation of the demographic structure resulting in relatively few larger oysters (Mann et al., Reference Mann, Southworth, Harding and Wesson2009a; Harding et al., Reference Harding, Mann, Southworth and Wesson2010; Southworth et al., Reference Southworth, Harding, Mann and Wesson2010) and reduced individual growth rates (Harding et al., Reference Harding, Mann and Southworth2008), whether from fishing, disease or selection pressures over decadal time scales, presents serious challenges for the maintenance of the oyster shell base (habitat) in natural populations. Maintenance of the shell base requires that natural shell degradation (30% per year: Powell & Klinck, Reference Powell and Klinck2007) be balanced by accretion (~3.5 mm year−1 in the Chesapeake region: Mann et al., Reference Mann, Harding and Southworth2009b). Actual habitat growth requires accretion at higher rates. To date, periodic years of extraordinary recruitment have maintained both the fishery and the shell base in the James River. In recent years the Great Wicomico (2004–2011) and Rappahannock Rivers (2000–2008) have experienced reduced harvest activity and focused shell planting efforts, which have maintained the resident oyster populations at modest levels. These efforts, combined with additional management strategies, will be required to sustain the resident oyster populations against the current backdrop of high mortality for larger/older oysters and the accompanying modifications in life history strategy.
ACKNOWLEDGEMENTS
This contribution is dedicated to the late Reinaldo Morales-Alamo for his numerous contributions to oyster biology during his 40 year career at the Virginia Institute of Marine Science. Erin Reilly assisted with field collections and laboratory analyses during summer 2008. Todd Nelson designed the hydrographic monitoring stations and assisted with their deployment. We thank the many individuals who have participated in autumn stock assessment surveys from 2006 through to 2009, particularly Dr James Wesson, Alan Godshall, Vernon Rowe, John Ericson, Adam Crockett, Erin Reilly and Matthew Robinson. Thanks are extended to Drs Eileen Hoffman and John Klinck for numerous constructive conversations. Funding was provided by the National Sea Grant Oyster Disease Research Program (V712120-ODU) and the Commonwealth of Virginia. This is contribution number 3215 from the Virginia Institute of Marine Science.
Supplementary materials and methods
The supplementary material referred to in this paper can be found online at journals.cambridge.org/mbi.



