Implications
Increased litter size has led to a decrease in average litter birth weight, consequently resulting in greater numbers of low birth weight piglets. Compared with their heavier littermates, low birth weight pigs display impaired growth efficiency and greater adipose tissue deposition. Because these traits are of primordial economic importance, low birth weight jeopardize a successful and efficient commercial pig production. The results of the present study revealed that, in order to overcome excessive adipose tissue deposition in the finisher period, low birth weight pigs should have only restricted access to feed.
Introduction
Over the last decade sow’s prolificacy markedly increased and as a consequence average birth weight decreased and displayed greater variability within litter (Quesnel et al., Reference Quesnel, Brossard, Valancogne and Quiniou2008; Campos et al., Reference Campos, Silva, Donzele, Oliveira and Knol2012). Responsible for this outcome are gestational factors such as intrauterine crowding and impaired placental development resulting in insufficient nutrient supply and therefore impaired foetuses development (Foxcroft et al., Reference Foxcroft, Dixon, Novak, Putman, Town and Vinsky2006; Wu et al., Reference Wu, Bazer, Wallace and Spencer2006). Because piglet’s survival rate during lactation is closely related to their birth weight (Quiniou et al., Reference Quiniou, Dagorn and Gaudré2002) and the percentage of piglets weighing <1 kg increases with increasing litter size (Bérard et al., Reference Bérard, Kreuzer and Bee2008; Campos et al., Reference Campos, Silva, Donzele, Oliveira and Knol2012), overall reproduction efficiency in terms of number of weaned piglets and total weaning weight might be compromised in high prolific sows. In case that low birth weight pigs survive the lactation period and reach the weaning age, there is compelling evidence that impaired foetal development negatively affects postnatal development (Bérard et al., Reference Bérard, Kreuzer and Bee2008; Beaulieu et al., Reference Beaulieu, Aalhus, Williams and Patience2010). Unanimously the results of the aforementioned studies showed that pigs born with a lower birth weight grew slower. In addition, negative relationships between birth weight and carcass fatness (Rehfeldt et al., Reference Rehfeldt, Kuhn, Fiedler and Ender2004; Gondret et al., Reference Gondret, Lefaucheur, Juin, Louveau and Lebret2006), drip loss (Rehfeldt and Kuhn, Reference Rehfeldt and Kuhn2006) and tenderness (Gondret et al., Reference Gondret, Lefaucheur, Juin, Louveau and Lebret2006; Bérard et al., Reference Bérard, Kreuzer and Bee2008) were reported.
Compensatory growth, a phenomenon of accelerated growth observed after a period of restricted feed supply has been known for decades. From a meat quality point of view the compensatory response is interesting, because it is believed that this process is mediated through an elevated protein turn over (Oksbjerg and Therkildsen, Reference Oksbjerg and Therkildsen2007). An inseparable part of the latter is proteolysis, which is partly regulated by the calpain system (Goll et al., Reference Goll, Neti, Mares and Thompson2008). As reviewed by Huff Lonergan et al. (Reference Huff Lonergan, Zhang and Lonergan2010), µ-calpain and its inhibitor calpastatin play an important role early postmortem and by that affect pork quality traits such as drip loss and tenderness. Because low birth weight has been associated with impaired water holding capacity (Rehfeldt and Kuhn, Reference Rehfeldt and Kuhn2006) and tenderness (Gondret et al., Reference Gondret, Lefaucheur, Juin, Louveau and Lebret2006; Bérard et al., Reference Bérard, Kreuzer and Bee2008), the objective of this study was to evaluate whether accelerated growth before slaughter caused by a compensatory growth response could be a suitable feeding strategy to alleviate the negative impact of low birth weight on pork quality.
Material and methods
Experimental design, animals and feeding
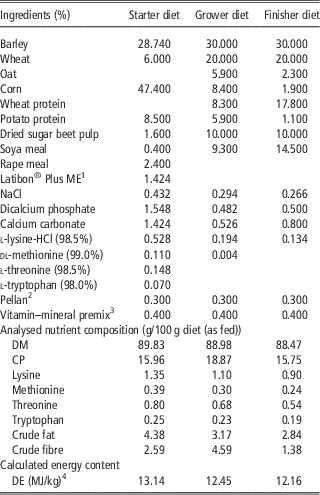
The Swiss Federal Committee for Animal Care and Use approved all procedures involving animals. From 21 litters, the lightest (L) and heaviest (H) barrows (Swiss Large White; n=42) were selected at weaning. A total of four successive farrowings, each 3 weeks apart, were needed to obtain the required number of pigs. In three farrowing groups six L and six H offspring and in one farrowing group only three L and three H barrows were selected from six and three sows, respectively. To be included in the study, the birth weight had to be in the range of >0.8 and <1.3 kg and >1.7 kg for L and H barrows, respectively. From weaning (mean±s.e.; 11.3±1.1 kg BW; 33±6 days of age) to the start of the grower period at 80±4 days of age, barrows were group penned (four to six pigs/pen) and given ad libitum access to the starter diet (Table 1). At the start of the grower period, H and L barrows of each farrowing group were moved to the grower–finisher stable and randomly assigned within birth weight group to one of three feeding regimes: AA: ad libitum access to the grower and finisher diet, RR: restricted access to the grower and finisher diet or RA: restricted access to the grower diet and ad libitum access to the finisher diet. In the grower and finisher period, pigs received the same grower and finisher diet (Table 1). Feed restriction, defined by the amount of feed, was designed to allow an average daily gain of 650 g/day from 27.8±0.7 to 102.1±1.1 kg BW. As outlined in the Swiss feeding recommendation for pigs (Agroscope Liebefeld Posieux Research Station (ALP), 2012) daily digestible energy (DE) intake was calculated based on the following equation: DE (MJ/day)=−0.37+65.23×(BW/100) −42.89×(BW/100)2+9.43×(BW/100)4. In the grower and finisher period, 18 and 24 barrows of the farrowing group one, two and three, four, respectively, were reared in two group pens (2.9 m2/pig). Each pen was equipped with two automatic feeders and individual pig recognition system (Schauer Agrotronic GmbH, Prambachkirchen, Austria) as described previously (Bee et al., Reference Bee, Guex and Herzog2004). Individual daily feed allowance as well as individual feed intake was monitored and recorded by the control software (MLP; SCHAUER) linked to each feeder. Because estimated DE content of the grower and finisher diet differed, daily and total intake of DE as well as DE energy intake per kg weight of each individual barrow was calculated by multiplying individual feed intake and DE content of the grower and finisher diet, respectively. Barrows were weighed weekly in the morning at 0700 h. Animals were not fasted before weighing. For those with restricted feed access, total daily feed allowance was adjusted weekly based on their individual BW. The week barrows reached ⩾60 kg BW, they were offered the finisher diet. This was done by using one of the two automatic feeders in the pen for the finisher diet and limiting the access only to the finisher pigs. Thus, until all barrows in the pen reached ⩾60 kg BW, one feeder was used for the grower and one for the finisher diet. The day after barrows reached 102 kg BW they were slaughtered. Before slaughter, barrows were fasted for 12 h. Slaughter and carcass dissection were carried out as described previously (Bee et al., Reference Bee, Guex and Herzog2004).
Composition of the experimental diets, as-fed basis

DM=dry matter; DE=digestible energy.
1 A multi-acid mixture used to improve acidity and promote antibacterial actions from foregut to hindgut.
2 Binder that aids in pellet formation.
3 Supplied the following nutrients per kg of diet: 20 000 IU vitamin A, 200 IU vitamin D3, 39 IU vitamin E, 2.9 mg riboflavin, 2.4 mg vitamin B6, 0.010 mg vitamin B12, 0.2 mg vitamin K3, 10 mg pantothenic acid, 1.4 mg niacin, 0.48 mg folic acid, 199 g choline, 0.052 mg biotin, 52 mg Fe as FeSO4, 0.16 mg I as Ca(IO)3, 0.15 mg Se as Na2Se, 5.5 mg Cu as CuSO4, 81 mg Zn as ZnO2, 15 mg Mn as MnO2.
4 DE content (MJ/kg) calculated from nutrient content (expressed in g/g DM) according to Agroscope Liebefeld Posieux Research Station (ALP) (2012).
Tissue sampling and preparation the day of slaughter
Within 30 min after exsanguination, the longissimus (LM) and semitendinosus (STM) muscles were removed from the right side of each carcass. Weight, girth and length of the STM and the LM area were determined after muscle excision. Muscle samples for histochemical analyses were excised from the centre of the dark portion of the STM (STMdark) and anterior to the 10th rib location of the LM. One piece (1×1×3 cm) of each muscle was immediately fixed on a labelled flat stick, rolled in talcum powder, immediately frozen in liquid nitrogen and stored at –80°C until histochemical analyses.
Meat quality traits
One day after slaughter, from the left carcass side two 1.5-cm thick LM chops were cut at the 12th rib level and two slices (∼70 g each) were obtained from the STMdark. From the muscle samples, pH and drip loss percentages were determined. At 30 min (from the right carcass side) and 24-h postmortem pH of the LM and STM was measured using a WTW pH meter (pH196-S; WTW, Weilheim, Germany) equipped with a WTW electrode (WTW Eb4; WTW) and a temperature probe. Drip loss percentage was measured as the amount of purge formed during storage of chops at 2°C for 24 and 48 h as a percentage of the initial chop weight (Honikel, Reference Honikel1998). After drip loss measurements were assessed, samples were vacuum-packed and stored at −20°C until Warner–Bratzler shear force was determined. Frozen samples were thawed for 24 h at 2°C, kept at room temperature for 1 h and then weighed. Cooking loss were measured as the amount of purge lost after cooking the chops on a grill plate (190 to 195°C; Beer Grill AG, Zurich, Switzerland) to an internal temperature of 69°C. Shear force was determined on the cooked samples previously cooled to ambient temperature using the original Warner–Bratzler device (model 3000; G-R Electric MFG Co., Manhattan, KS, USA). In the two LM chops, a total of eight cores of 1.27 cm diameter were obtained, whereas the STMdark were cut into eight strips of 10×10×50 mm. The maximum shear force for eight cores or strips per muscle sample, sheared across the fibre direction, was recorded and averaged for each sample.
Histochemical analysis
Histochemical procedures and determination of myofibre size and myofibre type distribution were carried out as described previously (Bee et al., Reference Bee, Guex and Herzog2004). Briefly, frozen LM and STMdark samples were equilibrated to −25°C, cut from the stick, and trimmed to facilitate transverse sectioning. In order to cut 10-µm-thick sections using a Cryotome (Shandon Inc., Pittsburgh, PA, USA), muscle samples were mounted on a cryostat chuck with a few drops of tissue-freezing medium (Tissue-Tek, Sakura Finetek Europe, Zoeterwoude, The Netherlands). Three sections, which were obtained within the muscle samples 30 µm apart, were mounted on glass microscopic slides and allowed to air-dry for 30 min. Subsequently, sections were treated with a combination of succinic dehydrogenase and acid myofibrillar ATPase, according to the multiple-staining procedure of Solomon and Montgomery (Reference Solomon and Montgomery1988). Stained sections were observed under transmitted light at a total magnification of 125× with an Olympus BX50 microscope (Olympus Optical Co., Hamburg, Germany) equipped with a high-resolution digital camera (ColorView12, Soft Imaging System GmbH, Munster, Germany). Based on the staining reaction, myofibres were classified into slow glycolytic (SO=dark staining), fast oxidative-glycolytic (FOG=intermediate staining) and fast glycolytic (FG=light staining). One random field within each of the three cryo-sections of a slide of each muscle sample was captured with the high-resolution digital camera, and a minimum of 250 myofibres per field (total per muscle sample: >750 myofibres) were analysed with the analySIS 3.0 image analysis software (Soft Imaging System GmbH). To minimize the incidence of measuring intrafasicular terminations of myofibres in the LM and STMdark, only myofibres larger than 700 µm2 were included in calculations. Myofibre type distribution was calculated as the percentage of each myofibre type to the total of all myofibres measured.
Myosin heavy chain isoform distribution in the LM muscle
Quantitative real-time PCR (RT-PCR) was performed on seven porcine genes: MyHC embryonic, MyHC perinatal, MyHC slow/I, MyHC IIA, MyHC IIX, MyHC IIB and β-actin. Each cDNA template for RT-PCR was prepared from mRNA extracted from 50 mg of LM tissue collected within 30 min after exsanguination (Trifast, Peqlab Biotechnologie GmbH, Erlangen, Gemany), by first-strand reverse transcription using 0.50 μg of oligo-d(T) (Improm-II reverse transcriptase, Promega, Mannheim, Germany) in a final volume of 20 µl. All used primers and taqman probes (Supplementary Table S1) are published by da Costa et al. (2002). The TaqMan PCR assays for each target gene were performed in triplicate on cDNA templates with a Rotor-Gene 6500 QRT-PCR thermocycler analyser (Corbett Life Science, Sydney, Australia) according to the manufacturer’s recommendations. For each cDNA sample, diluted 1 : 100, an amplification plot was generated, displaying an increase in the reporter fluorescence dye (ΔRn) with each PCR cycle. Each C t value (threshold cycle) was determined from the mean of three separate RT-PCR experiments. Relative standard curves for each gene were plotted showing C t (y-axis) v. log (initial cDNA) diluted 10-fold sequentially (x-axis). The cDNA used to generate the relative standard curves was from the ST muscle of a barrow not included in the study and slaughtered at a similar age and BW as the experimental animals. When PCR amplification is maximally efficient, resulting in a doubling of product in every cycle, the slope will be −3.3 (Medhurst et al., Reference Medhurst, Harrison, Read, Campbell, Robbins and Pangalos2000). In the present study, the mean slope of the six genes was −3.37±0.25.
The relative standard curve method was used to quantify the relative gene expression of embryonic, perinatal, slow/I, IIA, IIX, IIB MyHC isoforms and of β-actin as described by da Costa et al. (Reference da Costa, Blackley, Alzuherri and Chang2002). To correct for variations in the quality and quantity of cDNA templates, all MyHC isoform expression results were normalized to corresponding endogenous β-actin mRNA levels, which within each muscle were not affected by treatment (P⩾0.42).
DNA and RNA concentration in the LM and STMdark
Muscle samples of the LM and STMdark collected within 30 min after exsanguination were assayed for DNA and RNA concentration as described by Oksbjerg et al. (Reference Oksbjerg, Petersen, Sorensen, Henckel, Vestergaard, Ertbjerg, Moller, Bejerholm and Stoier2000). The DNA content was measured fluorometrically by a picogreen dsDNA quantitation reagent kit (Quant-iT™ PicoGreen® dsDNA Assay Kit, P7589, Life Technologies Europe B.V., Zug, Switzerland). The RNA was determined fluorometrically using a SybrGreen gel staining kit (SYBR® Green II RNA Gel Stain, S7568, Life Technologies Europe B.V.). The average RNA : DNA ratio within feeding strategy and birth weight group was calculated from the RNA : DNA ratios obtained from each individual muscle sample.
Statistical analysis
Data were analysed with PROC MIXED of SAS (Version 9.1, SAS Institute Inc., Cary, NC, USA) with the individual pig as the experimental unit. The model used for the data analyses of growth performance, carcass characteristics, meat quality traits, histological and RT-PCR data included feeding regime, birth weight group and the feeding regime×birth weight group interaction as fixed effects, and litter of origin as the random effect. For the variables average daily gain, daily and total intake of DE as well as DE energy intake per kg daily gain, pen and initial BW at the start of the grower period was included as fixed factor and covariate, respectively, in the statistical model. Least square means were calculated and the PDIFF option of SAS was used to determine differences between dietary treatment groups. Differences were considered as significant if P<0.05 and as tending to be significant if P<0.10.
Results
Growth performance, carcass characteristics and muscle morphometry
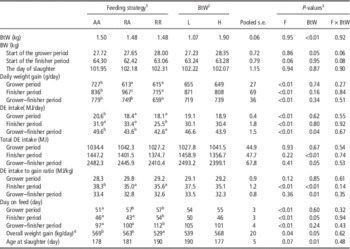
At birth, L barrows were 0.83 kg lighter (P<0.01) than H barrows (Table 2). Regardless of the applied feeding strategy (feeding strategy×birth weight group interaction; P>0.05), average daily weight gain in the grower–finisher period did not (P=0.34) differ but total DE intake and, therefore DE intake per kg weight gain, was greater (P⩽0.05) in L than H barrows. The aforementioned differences resulted from a greater (P⩽0.04) daily and total DE intake and impaired (P<0.01) DE efficiency in the finisher but not grower period. Compared with H, daily weight gain from birth to slaughter was lower (P=0.05) in L barrows and consequently these pigs were on average 13 days older (P=0.01) at slaughter.
Effects of three feeding strategies on growth performance of low and high BtW barrows

DE=digestible energy.
a,bValues within a row are different if superscript differs (P<0.05).
1 AA=ad libitum access to the diet during the growth and finishing period (n=14); RA=restricted and ad libitum access to the diet during the growth and finishing period, respectively (n=14); and RR=restricted access to the diet during the growth and finishing period (n=14).
2 H=high BtW (n=21); L=low BtW (n=21).
3 Probability values for feeding strategies (F), birth weight (BtW) and F×BtW interaction.
4 Calculated from BW at birth to BW at slaughter.
From the start of the grower period to slaughter, barrows of the AA and RA group grew faster (P<0.05) than RR barrows. Because average daily weight gain and average daily intake of DE differed to a similar extent in AA and RA compared with RR barrows, DE efficiency was similar (P>0.10) in the three feeding groups. During the compensatory growth period when feed allowance was switched from restricted to ad libitum, RA barrows grew faster (P<0.05) than AA or RR barrows despite daily DE intake was similar (P>0.10) for barrows with ad libitum feed allowance but greater (P<0.05) than for RR barrows. In contrast, DE intake per kg weight gain did not differ between RA and RR barrows but was lower (P<0.05) than for AA barrows. As expected, growth rate from birth to slaughter was lower (P<0.05) in RR compared with AA and RA barrows. The AA and RA barrows tended (P<0.10) to be 12 and 9 days younger at slaughter than RR barrows.
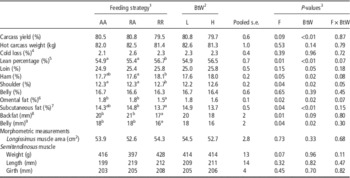
Compared with H barrows, the carcass yield was greater (P<0.01) in L barrows at the similar (P=0.14) carcass weight (Table 3). However, their carcasses were fatter as indicated by the lower (P⩽0.05) percentage lean meat including all primal cuts and greater (P⩽0.02) percentage omental and subcutaneous fat. The percentage lean meat and that of the ham and shoulder were lower (P⩽0.05) in AA and RA than RR barrows. These differences tended to be greater (feeding regime×birth weight group interaction; P⩽0.08) in L than H barrows. Regardless of the birth weight, the STM of RR barrows tended (P<0.10) to be heavier than the STM of AA and RA barrows. By contrast, the girth of the STM and the LM area were neither affected by the feeding regimen (P⩾0.32) nor the birth weight (P⩾0.33).
Effects of three feeding strategies on carcass characteristics and morphometric muscle measurements of low and high BtW barrows

a,bValues within a row are different if superscript differs (P<0.05).
1 AA=ad libitum access to the diet during the growth and finishing period (n=14); RA=restricted and ad libitum access to the diet during the growth and finishing period, respectively (n=14); and RR=restricted access to the diet during the growth and finishing period (n=14).
2 H=high BtW (1.94 kg; n=21); L=low BtW (1.07 kg; n=21).
3 Probability values for feeding strategies (F), birth weight (BtW) and F×BtW interaction.
4 Weight loss of the hot carcass during cooling at 2°C for 24 h.
5 Sum of denuded shoulder, back and ham weights as percentage of cold carcass weight.
6 Omental fat weight expressed as percentage of cold carcass weight.
7 Sum of external fat from the shoulder, back and ham expressed as percentage of cold carcass weight.
8 Backfat thickness determined at the 10th rib location.
9 Fat thickness determined at the 10th rib location.
Meat quality
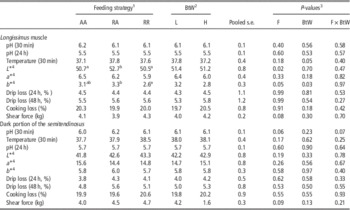
The impact of birth weight on meat quality traits was limited to the greater (P=0.05) LM temperature at 30-min postmortem and greater (P=0.03; higher b* values) yellowness of the LM of L barrows (Table 4). In addition, 30 min pH tended (P<0.10) to be greater in the STMdark of RA compared with AA barrows, with intermediate values for RR barrows. Regarding the effect of feeding strategy on pork quality, the LM of RA barrows was lighter (P<0.05; greater L* value) and more yellow (P=0.05) than the LM of AA and RR barrows. Shear force values tended (P<0.10) to be greater in both muscles of RR barrows compared with the LM of RA and the STM of AA barrows, respectively. None of the interactions for the pork quality traits were statistically significant.
Effects of three feeding strategies on meat quality traits of the longissimus muscle and dark portion of the semitendinosus muscle of low and high BtW barrows

a,bValues within a row are different if superscript differs (P<0.05).
1 AA=ad libitum access to the diet during the growth and finishing period (n=14); RA=restricted and ad libitum access to the diet during the growth and finishing period, respectively (n=14); and RR=restricted access to the diet during the growth and finishing period (n=14).
2 H=high BtW (1.94 kg; n=21); L=low BtW (1.07 kg; n=21).
3 Probability values for feeding strategies (F), birth weight (BtW) and F×BtW interaction.
4 L*=a measure of darkness to lightness (higher L* values indicates a lighter colour); a*=a measure of redness (higher a* value indicates a redder colour); and b*=a measure of yellowness (higher b* value indicates a more yellow colour).
DNA and RNA concentrations, myofibre characteristics and gene expression of MyHC isoforms in the LM and STMdark
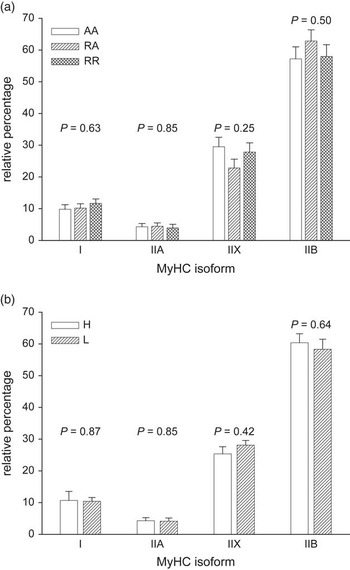
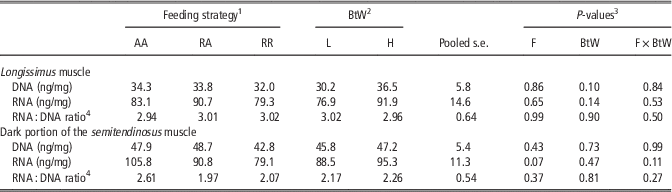
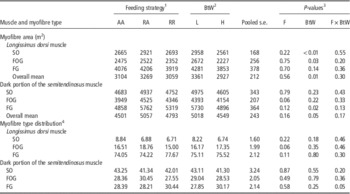
The DNA concentration in the LD but not the STMdark tended (P=0.10) to be lower in L than H barrows (Table 5). The RNA level and the RNA/DNA ratio in both muscles did not differ between the H and L birth weight group. In the STMdark, but not the LM, barrows of the RR treatment tended (P=0.07) to have lower RNA levels compared with AA and RA barrows. The DNA concentration and the RNA/DNA ratio in both muscles were similar for AA, RA and RR barrows. In L barrows, the SO, FOG and overall mean size of myofibres of the LM and the FG and overall mean size of myofibres of the STMdark were larger (P⩽0.03) than in H barrows (Table 6), whereas birth weight had no (P⩾0.18) effect on myofibre type distribution. The feeding regime did neither (P⩾0.11) affect myofibre size nor myofibre distribution, except for the FOG myofibres. The FOG myofibres of the STMdark tended (P<0.10) to be larger and the percentage of FOG fibres in the LM tended (P<0.10) to be greater in RA than in AA and RR barrows, respectively. RT-PCR showed that the highest mRNA levels were of MyHC IIB followed by IIX, I and IIA (Figure 1a and b). Neither, birth weight group (P⩾0.42) nor feeding regime (P⩾0.25) had an impact on relative levels of MyHC I, IIA, IIX and IIB transcripts.
Relative mRNA expression of myosin heavy chain (MyHC) isoform I, IIA, IIX and IIB determined in the longissimus dorsi muscles. Panel a depicts the results of the three feeding strategies (AA=ad libitum access to the diet during the grower–finisher period (n=14); RA=restricted and ad libitum access to the diet during the grower and finisher period, respectively (n=14); and RR=restricted access to the diet during the grower–finisher period (n=14)) and panel b depicts the results of the high (H=1.94 kg BW; n=21) and low (L=1.07 kg BW; n=21) birth weight group. Columns and error bars represent least squares means and s.e. The P-values reported for each isoform represent the effect of feeding strategy (a) and birth weight (b). Feeding×birth weight interaction was not significant.

Effect of three feeding strategies on the DNA and RNA concentration as well as RNA : DNA ratio determined in the longissimus muscle and dark portion of the semitendinosus muscle of low and high BtW barrows

1 AA=ad libitum access to the diet during the growth and finishing period (n=14); RA=restricted and ad libitum access to the diet during the growth and finishing period, respectively (n=14); and RR=restricted access to the diet during the growth and finishing period (n=14).
2 H=high BtW (1.94 kg; n=21); L=low BtW (1.07 kg; n=21).
3 Probability values for feeding strategies (F), birth weight (BtW) and F×BtW interaction.
4 The average RNA : DNA ratio was calculated from the RNA : DNA ratios obtained from each individual muscle sample.
Effects of three feeding strategies on myofibre area and myofibre type distribution in the longissimus muscle and dark portion of the semitendinosus muscle of low and high BtW barrows

SO=slow oxidative; FOG=fast oxidative-glycolytic; FG=fast glycolytic.
1 AA=ad libitum access to the diet during the growth and finishing period (n=14); RA=restricted and ad libitum access to the diet during the growth and finishing period, respectively (n=14); and RR=restricted access to the diet during the growth and finishing period (n=14).
2 H=high BtW (1.90 kg; n=21); L=low BtW (1.07 kg; n=21).
3 Probability values for feeding strategies (F), birth weight (BtW) and F×BtW interaction.
4 Myofibre type distribution expressed as the percentage of each myofibre type to the total of all myofibres measured.
Discussion
Worldwide there is strong economic incentive to increase litter size as well as number of yearly weaned piglets per sow. Improvement of the reproductive performance can only be realized with highly prolific sow lines. The consequence of increased litter size is reduced intrauterine space per foetus, also known as intrauterine crowding, resulting in intrauterine growth retardation and ultimately low birth weight (Bérard et al., Reference Bérard, Pardo, Bethaz, Kreuzer and Bee2010b). Lower birth weight of piglets is not only associated with reduced likelihood of pre-weaning and nursery survival (Fix et al., Reference Fix, Cassady, Holl, Herring, Culbertson and See2010) but also impaired growth efficiency and unfavourable carcass characteristics (Rehfeldt et al., Reference Rehfeldt, Kuhn, Fiedler and Ender2004; Gondret et al., Reference Gondret, Lefaucheur, Juin, Louveau and Lebret2006; Bérard et al., Reference Bérard, Kreuzer and Bee2008). Because the percentage of piglets with rather low birth weight increases with increasing litter size, overall efficiency of pig production might therefore be lowered. In light of these facts, it seems relevant to evaluate whether alternative feeding strategies might alleviate the reduced production efficiency. The major finding of the present study is that the prenatally imprinted negative characteristics of low birth weight barrows cannot be overcome during postnatal growth by using the compensatory growth strategy in the finisher period.
Effects of birth weight
In the present study and in line with earlier results (Gondret et al., Reference Gondret, Lefaucheur, Juin, Louveau and Lebret2006; Rehfeldt and Kuhn, Reference Rehfeldt and Kuhn2006; Bérard et al., Reference Bérard, Kreuzer and Bee2008), impaired growth efficiency in the grower–finisher period became manifested in the greater amount of ingested DE, impaired DE efficiency and more days on feed of L compared with H barrows. As observed by Bérard et al. (Reference Bérard, Kreuzer and Bee2010a), daily weight gain was lower from birth to slaughter but not in the grower–finisher period. This implies that growth rate and consequently age differences at slaughter between the two birth weight groups resulted primarily from the pre- and post-weaning period. During the lactation period, increased milk intake, due to the greater ability of heavier littermates to reach, occupy, stimulate and drain the best performing teats of the dam, results in greater growth and ultimately greater weaning weights (Quiniou et al., Reference Quiniou, Dagorn and Gaudré2002). As shown previously by Bérard et al. (Reference Bérard, Kreuzer and Bee2010a), in the post-weaning period weight gain difference seems to stand because, when placed in collective pens and feed was offered ad libitum, heavier piglets ingested more DE than lighter piglets. However, interestingly the current results suggested that regardless of the applied feeding strategy, the impact of birth weight decreased with increasing age. However, Gondret et al. (Reference Gondret, Lefaucheur, Juin, Louveau and Lebret2006) reported greater growth rates of high compared with low birth weight pigs not only in the suckling and post-weaning but also in the grower–finisher period. Possible reasons for this discrepancy might be the nutrient composition of the finisher diet and the rearing conditions. Gondret et al. (Reference Gondret, Lefaucheur, Juin, Louveau and Lebret2006) used in their experiment a finisher diet, which was richer in CP, crude fat and energy. Furthermore, in their study barrows were reared in individual and not in group pens resulting in an overall greater daily energy intake due to lack of animal to animal interaction. Both factors might have limited full expression of growth potential of the H barrows in the present study.
A consequence of the lower feed efficiency, adipose tissue deposition was greater in L compared with H barrows, which matches results of previous studies (Gondret et al., Reference Gondret, Lefaucheur, Louveau, Lebret, Pichodo and Le Cozler2005). Gondret et al. (Reference Gondret, Lefaucheur, Juin, Louveau and Lebret2006) found elevated lipogenic enzyme activities, greater lipid content and larger adipocytes in the adipose tissue of low compared with high birth weight female pigs slaughtered at the same weight. Interestingly, at day 75 of gestation it appears that differentiation of adipose tissue and maintenance of preadipocyte state depends on foetal development as mRNA levels of preadipocyte-related genes were greater in the subcutaneous backfat of small compared with large foetuses (Gondret et al., Reference Gondret, Perruchot, Tacher, Bérard and Bee2011). In line with these observations, small piglets did possess more adipocytes than their normal-sized and large siblings on postnatal day 7 (Williams et al., Reference Williams, Marten, Wilson, Litten-Brown, Corson, Clarke, Symonds and Mostyn2009), and a greater density of small-sized adipocytes on postnatal day 14 when compared with controls (Attig et al., Reference Attig, Djiane, Gertler, Rampin, Larcher, Boukthir, Anton, Madec, Gourdou and Abdennebi-Najar2008). The latter indicates greater proliferation of fat cells in low birth weight pigs as an adaptive phenomenon designed to improve long-term capacity for lipid storage, for example, during the lactation period, where feed supply is restricted. However, after weaning feed was available ad libitum and previous fat cell hyperplasia promoted excess adiposity. In the current study, fat cell number was not assessed but the observed greater adiposity of the L barrows might be explained by the aforementioned mechanism.
The greater percentage of adipose tissue in low compared with high birth weight pigs might also be due to differences in pre- and postnatal muscle development (Rehfeldt and Kuhn, Reference Rehfeldt and Kuhn2006). Ward and Stickland (Reference Ward and Stickland1991) concluded that in pigs myofibre hyperplasia is completed by day 90 of gestation, whereas recent data suggest that naturally or due to dietary interventions a certain increase in myofibre number occur within the first weeks of life (Lösel et al., Reference Lösel, Kalbe and Rehfeldt2009; Bérard et al., Reference Bérard, Kalbe, Lösel, Tuchscherer and Rehfeldt2011). Nevertheless, the available data unequivocally show that at birth low birth weight pigs have fewer myofibres but of greater size compared with their higher birth weight littermates (Pardo et al., Reference Pardo, Bérard, Kreuzer and Bee2013). In this study, mean myofibre size was 15 and 10% greater in the LM and STMdark, respectively, in L barrows but no morphometric changes in muscle characteristics were observed. This leads to the assumption that the two muscles of L barrows contained fewer myofibres at slaughter. These findings confirm previous observations suggesting that differences at least in myofibre number and size at birth persist until the day of slaughter (Gondret et al., Reference Gondret, Lefaucheur, Juin, Louveau and Lebret2006). Thus, during postnatal growth maximal myofibre hypertrophy might be attained earlier in low compared with high birth weight pigs and therefore, as suggested by Rehfeldt and Kuhn (Reference Rehfeldt and Kuhn2006), dietary energy cannot longer be used for muscle protein accretion but will be diverted to adipose tissue accretion. In accordance, indicators of satellite cell proliferation and of protein synthesis capacity were lower in the LD (by trend for DNA and numerically for RNA) in L than H pigs.
Meat quality traits were only marginally affected by birth weight, which confirms results of other experiments (Bérard et al., Reference Bérard, Kreuzer and Bee2008 and Reference Bérard, Kreuzer and Bee2010a; Beaulieu et al., Reference Beaulieu, Aalhus, Williams and Patience2010). However, others observed greater drip loss (Rehfeldt and Kuhn, Reference Rehfeldt and Kuhn2006) and lower sensory scores for tenderness (Gondret et al., Reference Gondret, Lefaucheur, Juin, Louveau and Lebret2006) in meat from low birth weight pigs. Using crossbred (Large White×Landrace) sows and pure Piétrain boars, Gondret et al. (Reference Gondret, Lefaucheur, Juin, Louveau and Lebret2006) reported a negative relationship (−0.338) between average myofibre size of the LM and tenderness scores, whereas in the present study in both muscles no significant relationships were detected between shear force values and the SO, FOG, FG and overall mean myofibre size. A possible explanation for the contradictory findings could be that regardless of birth weight, average myofibre size was 53% smaller in the current compared with the study of Gondret et al. (Reference Gondret, Lefaucheur, Juin, Louveau and Lebret2006) (6643 v. 3144 µm2). Thus, the impact of birth weight might differ depending on myofibre size, the latter being markedly different among breeds.
Effects of compensatory growth feeding strategy
As expected, in the finisher period fastest growth rate was observed in RA barrows. When compared with RR barrows, compensatory growth of RA barrows appeared to be linked to greater muscle protein synthesis because RNA levels were greater in the STMdark by trend and were numerically greater in the LD. Despite lacking statistical significance, the present data are in agreement with results reported by Oksbjerg et al. (Reference Oksbjerg, Sorensen and Vestergaard2002). Interestingly, for the growth performance traits there was no feeding strategy×birth weight category interaction indicating that the compensatory growth effect was similar for L and H pigs. In the finishing phase, a period known to exhibit increased fat deposition rate especially in barrows, lower feed efficiency corroborates with the lower carcass lean meat percentage of RA and AA pigs. The fact that low birth weight pigs have fewer adipocytes present for lipid filling (Attig et al., Reference Attig, Djiane, Gertler, Rampin, Larcher, Boukthir, Anton, Madec, Gourdou and Abdennebi-Najar2008; Williams et al., Reference Williams, Marten, Wilson, Litten-Brown, Corson, Clarke, Symonds and Mostyn2009) might explain that ad libitum feed access exhibited to a greater extent the full expression of lipogenic potential and ultimately fat growth in low compared with high birth weight littermates. On the other hand, restricted feed access and consequently lower dietary energy intake prevented excessive adipose tissue accumulation as carcass composition of low and high birth weight littermates displayed a comparable percentage of lean and adipose tissue. Therefore, as far as body composition and feed efficiency are considered, one could conclude that restricting dietary energy intake is the feeding strategy of choice for low birth weight pigs.
Acknowledgements
The authors would like to thank Bernard Dougoud and Guy Maikoff for their excellent technical assistance.
Supplementary material
To view supplementary material for this article, please visit http://dx.doi.org/10.1017/S1751731114002663