


1. Introduction
A. L. Hodgkin and A. F. Huxley's (Reference Hodgkin and Huxley1952) quantitative model of the action potential (HH model henceforth) is widely seen as a landmark achievement in neuroscience. For philosophers of science, it provides a rich and revealing case study for examining issues about explanation and causation, as well as the role of experimentation and physical theory in neuroscience. Fortunately—for the purpose of debate—different authors have given totally divergent philosophical accounts of this case. In Weber (Reference Weber2005, Chapter 2), I have argued that this model is a paradigm case of a biological phenomenon explained by physical-chemical laws. I have defended a thesis of explanatory heteronomy, which states that the explanatorily relevant generalizations in this case are nonbiological. The role of the biological concepts that are involved in this case (e.g., the concept of neuron) is to pick out the class of systems and to determine the relevant boundary conditions that feature in an otherwise purely physical-chemical explanation.
By contrast, Bogen (Reference Bogen2005) has defended a nonexplanatory account of the HH equations. On his view, these equations do describe regularities, but these regularities are not constitutive for causal relations. Unlike regularity theorists of causation who believe that they are conceptually linked, Bogen thinks that causal relations and regularities sometimes come apart. On his view, regularity theories of causation have diverted philosophers from other important functions of regularities in science. In particular, regularities play important epistemic or investigative roles. Regularities can summarize and systematize many years worth of experimental work. As such, they can point investigators to facts that need to be explained and to the workings of the underlying mechanisms. It is these mechanisms that are doing the explanatory work; the regularities are merely tools for their discovery. I absolutely agree with Bogen that regularities such as the ones contained in the HH equations play important epistemic roles other than explanation. However, as I will show here, the fact that the HH model summarized, in a systematic way, a large number of experiments does not exclude that it also had explanatory force.
A third philosophical account of the HH model is found in Craver (Reference Craver2007, Reference Craver2008). Craver argues that the HH model is at best a sketch of an explanation that, by itself, does not explain anything but that cleared the ground for a mechanistic explanation. For a mechanistic explanation à la Craver, scientists need to be able to label the nuts and bolts of a mechanism, to be precise, its entities and activities. Hodgkin and Huxley were not yet able to do so; only once the ion channels that carry the membrane currents were characterized biochemically was there an explanation of the action potential. In contrast to Bogen, Craver grants the HH model some explanatory value, however. On his view, the model provided a how possibly explanation rather than a how actually explanation. In other words, it provided a space of possible mechanisms that could produce the phenomena in question rather than showing how neural membranes actually generate action potentials.
In this article, I will defend the view that the HH model gave a causal explanation of action potentials against Craver's and Bogen's views. I will also defend the explanatory heteronomy thesis and examine further the interplay of physical laws and experimental generalizations. In the following section, I shall provide an in-depth analysis of the model. In Section 3, I show that it satisfies two important criteria for causal models: invariance and modularity in the sense of Woodward (Reference Woodward2003). In Section 4, I examine the roles that experimental generalizations and physical laws play in this example. A comparison with a very simple example from physics will demonstrate that the explanatory heteronomy thesis with respect to the HH model is correct. Section 5 summarizes my conclusions.
2. Analysis of the HH Model
The core of the HH model is the so-called total current equation that gives the total transmembrane current as a function of the membrane capacitance (C M), voltage (V), the equilibrium potentials for sodium and potassium (V Na and V K, respectively), the maximum conductances for sodium and potassium ( $\overline{g}_{\mathrm{Na}\,},\,\overline{g}_{\mathrm{K}\,}$) and the so-called gating variables n, m, and h (Hodgkin and Huxley Reference Hodgkin and Huxley1952, 518):Footnote 1

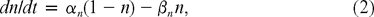


The sum in (1) contains terms for the capacitance current, potassium current, sodium current, and leak current (in this order). The capacitance current is proportional to the first time derivative of the transmembrane voltage, whereas the potassium and sodium currents are functions of the gating variables and of voltage. The equilibrium or rest potentials (V K, V Na) are given by the Nernst equation for each ion species r:

where T is temperature, R and F the gas and Faraday constants, and c o and c i are ion concentrations at the outside and inside of the membrane, respectively. The importance of the Nernst equation is that it gives the ion-motive force for each ionic species, which is proportional to the difference between actual potential and equilibrium potential:

The gating variables follow first-order differential equations and contain flux rate variables designated by Greek symbols (eqq. [2] –[4]). These rate variables are functions of voltage, but not of time. Hodgkin and Huxley obviously fitted them to the experimentally determined curves (Reference Hodgkin and Huxley1952, 519):


The potassium conductance term (the second summand in the total current eq. [1]) was given a physical interpretation by Hodgkin and Huxley (Reference Hodgkin and Huxley1952): “These equations [for sodium conductance and the gating variable n] may be given a physical basis if we assume that potassium ions can only cross the membrane when four similar particles occupy a certain region of the membrane. N represents the proportion of the particles in a certain position (for example, at the inside of the membrane) and  $1-n$ represents the proportion that are somewhere else” (507).
On this interpretation, the variables αn and βn express the rates of inward and outward flux of potassium ions, respectively. Similarly, the sodium term in (1) is also given a physical interpretation: “These equations [for potassium conductance and the gating variables m and h] may be given a physical basis if sodium conductance is assumed to be proportional to the number of sites on the inside of the membrane which are occupied simultaneously by three activating molecules but are not blocked by an inactivating molecule. m then represents the proportion of activating molecules on the inside and  $1-m$ the proportion on the outside; h is the proportion of inactivating molecules on the outside and
 $1-h$ the proportion on the inside” (Hodgkin and Huxley Reference Hodgkin and Huxley1952, 512). Just as before, αm, βh, βm, αh are interpreted as flux rates.
An integration of this equation gave a remarkable agreement with the records obtained from giant squid axon (Hodgkin and Huxley Reference Hodgkin and Huxley1952, 52). This must be one of the most accurate quantitative predictions of a biological phenomenon of all times.
In order to analyze the model, it is useful to divide it into two parts: (1) the conductance model and (2) the action model. The former consists of the equations for the potassium and sodium conductances (eqq. [2] –[4]) in conjunction with some equations that give the dependence of the flux rates on transmembrane voltage (eqq. [7] –[12]). The action model cannot be exhibited by merely pointing to some equations, but it forms an important part in the physical interpretation of the total current equation. I suggest that the following propositions are crucial for the action model (the following formulations are all quotations from the HH text):
i. Depolarization causes a transient increase in sodium conductance and a slower but maintained increase in potassium conductance. (500)
ii. These changes are graded and … can be reversed by repolarizing the membrane. (500)
iii. The changes of permeability appear to depend on membrane potential and not on membrane current. (501)
This suggests that what Hodgkin and Huxley were trying to establish is that a membrane with conductance properties as observed in actual experiments (summarized in the conductance model) generates action potentials with the right shape where the early voltage rise at the beginning is caused by the entry of Na+ and the later voltage fall is caused by the loss of K+. Furthermore, the model also shows that all this can happen in the absence of active ion translocation.
Craver and Bogen both emphasize (correctly) that the mechanism that Hodgkin and Huxley assumed for ion translocation was mistaken. Today, membrane permeability is thought to be controlled by selective ion channels. To be sure, Hodgkin and Huxley were aware that their presumed mechanism involving carrier particles for the ions (see the above quotations) was highly speculative. Further, they pointed out that different equations with different physical interpretations might have been equally successful in predicting action potentials:
The agreement [of the theoretical calculations and records of action potentials in squid axons] should not be taken as evidence that our equations are anything more than an empirical description of the time course of the changes in permeability to sodium and potassium. An equally satisfactory description of the voltage clamp data could no doubt have been achieved with equations of very different form, which would probably have been equally successful in predicting the electrical behavior of the membrane. … Certain features of our equations were capable of a physical explanation, but the success of the equations is no evidence in favour of the mechanism of permeability change that we tentatively had in mind when formulating them. (541)
Craver and Bogen take this passage as supporting their view that the HH model did not explain action potentials. However, this passage must be contrasted with the following one, which occurs on the same page: “The point that we do consider to be established is that fairly simple permeability changes in response to alterations in membrane potential, of the kind deduced from the voltage clamp results, are a sufficient explanation of the wide range of phenomena that have been fitted by solutions of the equations” (emphasis added).
Are Hodgkin and Huxley contradicting themselves? I suggest that their conclusions can be made consistent by reading “our equations” in the first quotation as referring to the conductance equations only, namely, the terms for sodium and potassium conductance. Indeed, it cannot be said that this physical interpretation was supported by the model's empirical success. The conductance equations were clearly fitted to the data; they are experimental generalizations.
However, I claim that none of this implies that the model as a whole was not explanatory, nor did Hodgkin and Huxley think so. Note that the propositions that I singled out as components of the action model are all expressed in causal language: depolarization causes a transient increase, permeability changes depend on membrane potential. I see no reason for doubting that when Hodgkin and Huxley say “causes,” they mean it. The model was clearly intended as a causal model. It is important to keep two tasks separate: (1) the identification of causal relations and (2) the physical basis or mechanism that is responsible for these causal relations. Hodgkin and Huxley succeeded on the first task, but they partially failed on the second. My account, therefore, does not contradict Hodgkin and Huxley's own assessment of their model.
An important contribution of Hodgkin and Huxley's was an experimental test of the emerging model of the action potential. This was a tricky business because of all the curve fitting that was going on. The two electrophysiologists were quite aware of this issue, as is evident in the opening paragraph of their discussion section: “This is a satisfactory agreement, because the equations and constants were derived entirely from ‘voltage clamp’ records, without any adjustments to make them fit the phenomena to which they were subsequently applied” (541). Here, I interpret Hodgkin and Huxley as saying that the data to which the equations were fitted were not taken from actual action potentials as they occur under physiological conditions. Rather, these data were obtained by measuring the electrical properties of the membranes under a variety of artificially induced conditions, in particular various ionic strengths on the inside and outside of the membrane and electrical fields applied from the outside (“voltage clamp”). Therefore, the successful prediction of action potentials with the right shape does constitute a test for the HH model. However, I suggest that this test only provided strong evidence for the action model. The conductance model was purely a result of curve fitting to which Hodgkin and Huxley tried to give a physical rationale later. But the conductance model was necessary in order to show that the assumptions of the action model would actually be able to generate action potentials with the right shape. It might seem remarkable that a model with a false physical interpretation should be part of a successful empirical test of another model that is essentially correct. We might have here another instance of how false models can lead to true theories (see Wimsatt Reference Wimsatt, Nitecki and Hoffman1987). I suggest, as a general rule, that a model M1 may be used to test another model M2 if M1's physical interpretation is independent of M2's causal content and if M1 gives the correct dynamics for a set of variables of M2. I want to maintain that, even though the HH model contained false mechanistic assumptions, it correctly described an abstract causal structure that is defined by the propositions i–iii mentioned above.
Note that none of these propositions were trivial or beyond doubt in 1952. The “sodium hypothesis” (Hodgkin and Katz Reference Hodgkin and Katz1949) explained how the action potential could be much larger than the resting potential. Under the well-known theory of nerve excitation of Bernstein (Reference Bernstein1912), this was puzzling. Bernstein had suggested that the membrane becomes permeable to all ions alike during the action potential. Therefore, the selective permeability changes to potassium and sodium are crucial for understanding how the potential could be so large (actually reversing the sign of the potential) on the basis of passive ion transport alone.
One could say that i–iii formed the causal content of the HH model. Hodgkin and Huxley were the first to work them into a comprehensive model of neural membrane behavior. They compose what I call the action model. By contrast, the conductance model, while its physical interpretation was false, was good enough to help showing that the causal content of the action model was able to generate action potentials (because it contained the right dynamics for these variables, even if the physical model of how this dynamics came about was false). In the following section, I will further investigate the causal-explanatory status of the model.
3. Experimental Regularities and Causation
In the previous section, I have shown that the HH model can be analyzed into two parts, the conductance and the action model. The former describes how membrane permeability depends on voltage. The latter shows how, given these permeability changes, a series of events takes place that are driven entirely by passive ion transport, that is, transport caused by differences in electrochemical potential across the neural membrane. In this section, I would like to examine further the status of the conductance model. Specifically, I want to apply a recent philosophical account of causal explanation, namely, Woodward's (Reference Woodward2003), to show that the HH model is an explanatory generalization.
The conductance model is an experimentally determined regularity concerning the conductance properties of neural membranes. In this respect, I fully agree with Bogen's (Reference Bogen2005) conclusion that the HH model summarizes a large amount of experimental data. I also agree with Craver (Reference Craver2006) that Hodgkin and Huxley did not know the mechanism responsible for the conductance changes. However, where I must part with both Bogen and Craver is in their assumption that these (uncontroversial) facts about the HH model imply that the model has no causal content. On the contrary, I would like to claim that the model is a beautiful case of an experimentally determined causal regularity.
According to Woodward (Reference Woodward2003, Chapter 6), generalizations can provide causal explanations to the extent in which they are invariant under certain interventions, namely, interventions on the independent variable(s) of the relationship. This invariance need not be total; causal generalizations may be invariant under some interventions but not others. (Only a few fundamental physical laws are invariant under any interventions.) I claim that Hodgkin and Huxley's total current equation (1) is invariant under at least some interventions. In particular, it continues to hold under interventions that alter the transmembrane voltage (e.g., in voltage clamp measurements) as well as the concentrations of potassium and sodium ions. So the total current equation qualifies as a causal explanatory generalization in Woodward's sense, even though it is not invariant under any intervention.
At this point, the following objection may be raised: the total current equation contains variables that do not seem to be subject to interventions, namely, the gating variables n, m, and h. These variables were purely fictional in 1952. The physical interpretation that Hodgkin and Huxley gave for them is false. They did not know why the membranes had the conductance properties that they observed.
However, I do not see why this should affect the HH model's explanatory status. Woodward's account does not say that all the variables in a causal relationship must be subject to interventions. It only says that there must at least be one independent variable that can be manipulated and that will change the value of the dependent variable in the way stated in the equation. The HH equations satisfy this condition. At least the transmembrane voltage V (this is what voltage clamp measurements actually manipulate), but also other variables (see above) can be manipulated in a way that changes the value of the dependent variable (current). The gating variables are part of the function that states exactly how the dependent variable changes under certain interventions. To do this, they need no correct physical interpretation.
Craver (Reference Craver2008) claims that the HH equations are purely phenomenological, sort of like epicycles in Ptolemaïc astronomy. They make correct predictions, but otherwise they are plainly false. I object to this analogy. Epicycles are not such that they can be replaced, within the framework of pre-Copernican astronomy, with some correct model or equation to give a true theory. By contrast, the HH model has exactly this property. First, the gating variables can be reinterpreted as properties of ion channels (Kuffler, Nicholls, and Martin Reference Kuffler, Nicholls and Martin1984, 149). If the relevant equations can be given a new interpretation so that they say something (approximately) true, then they must have gotten some salient causal relations right, even though their authors did not know the correct physical interpretation.
Second and perhaps more importantly, the HH model shows the property of modularity in Woodward's (Reference Woodward2003, 329) sense. For example, if potassium conductance is artificially increased by a potassium ionophore (an intervention in Woodward's sense), this will break the relationship  $g_{\mathrm{K}\,}=\overline{g}_{\mathrm{K}\,}n^{4}$ while leaving the other equations untouched. Modularity is thought to be necessary for equations to represent causal structures (Woodward Reference Woodward2003, 48). The HH equations thus satisfy all the conditions that a major recent theory of causation and explanation requires from causal-explanatory generalizations. There is simply no conflict between a generalization being causal and explanatory and its being an experimental generalization or being fitted to data. Experimentation is known to be a powerful way for finding out about causal relations, and this is what Hodgkin and Huxley did.
I have argued that the fact that Hodgkin and Huxley did not know what properties the gating variables expressed does not mean that they were not part of a causal regularity. In this context, it is worth noting that there are many causal regularities in physics and biology where it is not known exactly what mechanism is responsible for them. For example, classical geneticists in the early twentieth century knew some causal regularities concerning the transmission of hereditary factors in sexually reproducing organisms, for example, Mendel's laws and all the associated generalizations of classical genetics. Further, they were able to pinpoint the actual difference-making causes of some traits rather precisely to certain chromosomal locations, for example, the causes that make the difference between red- and white-eyed flies in laboratory populations of the fruit fly Drosophila.Footnote 2 Yet classical geneticists did not know the mechanism by which these chromosomal regions produce this effect. In fact, this was only solved very recently: the Drosophila white gene encodes a membrane transport protein that seems to affect the deposition of pigment in the eyes. This was totally unexpected, yet we would not say that classical geneticists had no causal knowledge. If we allow only mechanistic explanations in the sense of Machamer, Darden, and Craver (Reference Machamer, Darden and Craver2000) or Craver (Reference Craver2006, Reference Craver2007) as causal explanations, then causal explanations are quite scarce.
4. Explanatory Heteronomy: Will the Laws of Physics Please Stand Up
In the previous section, I have focused on the experimental generalizations that describe the conductance changes in neuronal membranes. In this section, I shall discuss the role of physical laws in the HH model. To this purpose, it will be useful to compare the HH model to a very simple example from physics. The example is actually taken from Woodward (Reference Woodward2003, 13).
Consider a rigid block of mass m sliding down an inclined plane at an angle φ. The motion of this block can be explained by the gravitational force that acts on the block, which points toward the Earth's center of mass and amounts to  $F_{g}=mg$, where g is the gravitational potential. Further, the block will experience a frictional force that is directed in the opposite direction with respect to its motion and that amounts to
 $F_{k}=\mu _{k}N$, where μk is the coefficient of friction and N the normal force exerted by the plane. The forces must be added, taking into account the angle of inclination, φ. This gives

for the net force and, due to the equivalence of gravitational and inertial mass,

for the acceleration. Woodward uses this case to illustrate his theory of causal explanation. The last identity expresses an invariant generalization that holds over a range of the variables m and φ. This means that there are patterns of counterfactual dependence involving different values of these variables. The variables are intervention variables, which roughly means that manipulating these variables will change the dependent variable a via a route that does not alter any other variable that is causally relevant for a (i.e., the salient counterfactuals are nonbacktracking in David Lewis's sense).
I take it that this is an uncontroversial case of a causal explanation. However, note that the simple model discussed by Woodward makes no assumption about the mechanisms responsible for the frictional force. The equation  $F_{k}=\mu _{k}N$ is an experimental generalization. To explain why it holds over a certain range of normal force for certain materials will involve some rather heavy physics (probably quantum mechanics will have to come into play). The coefficient of friction is an empirically determined magnitude. While it might be possible to theoretically calculate the coefficient of friction for certain materials, using fundamental physical theories, this is not necessary to give a causal explanation for why a block slides down an inclined plane at a certain acceleration. To be sure, such a fundamental physical account of friction would greatly enrich our understanding for specific cases (as the discovery of ion channels enriched neuroscientific explanations). But this does not mean that the more superficial model provides no causal explanation at all. In fact, the superficial model has a nice generality to it, as it applies to very different materials, abstracting from the details of their molecular structure.Footnote 3 This is what physical explanations often do.
I suggest that the HH model shares some features of the simple physical model just discussed: it combines fundamental physical laws (e.g., Newton's laws or Coulomb's law) with experimentally determined regularities that summarize the behavior of some physical object. What I have termed the HH conductance model is such an experimental generalization. The gating variables h, m, and n are analogous to the coefficient of friction in Woodward's example. They summarize the experimentally determined behavior of a physical object in a causal regularity. At the same time, the HH model as well as Woodward's block-on-an-inclined-plane model incorporate fundamental principles of physics to explain the behavior of the object under study. Thereby, they reduce the number of brute facts we have to accept.Footnote 4 In Woodward's example, the fundamental principles include Newton's laws. In our present neuroscientific example, the most fundamental physical principle is the Nernst equation, which is derivable ab initio, in combination with relationships that determine ion-motive forces (6). It's these forces that move the ions about in the nervous system. Thus, the HH model provides a causal explanation that is characteristic of much macrophysics.
The analogy to a simple physical example also demonstrates the essential correctness of the explanatory heteronomy thesis (Weber Reference Weber2005).Footnote 5 In Woodward's example, no one would doubt that it is merely an application of physical principles to a special type of system, in this case systems that exhibit gravitational and frictional forces as specified in the model. The HH model is no different in this respect. It applies fundamental physical principles, namely, the Nernst equation. At the same time, it contains experimentally determined regularities that are not derivable from fundamental physical laws but that are needed to apply the latter to a specific type of system. But even thought these regularities are not themselves derived from more fundamental laws, they describe causal structures.
5. Conclusions
The HH model shows an entwinement of experimental regularities and fundamental physical laws that is typical of physical explanations. Such explanations often abstract from the detailed mechanisms that realize some physical properties, without thereby being rendered noncausal. The same is true for many explanations in the special sciences, for example, genetics. As for the thesis of explanatory heteronomy (Weber Reference Weber2005, Chapter 2), it appears to be defensible for this case: the explanatory principles contained in the HH model are either derivable ab initio (specifically, the Nernst equation) or they represent experimental generalizations involving physical properties such as voltage and conductance that describe causal structures to which the fundamental laws are applied. I have shown that the HH model exhibits the two properties of invariance and modularity, which a major recent theory of causal explanation holds to be crucial. Mechanisms in the narrow sense much discussed in recent philosophy of biology and neuroscienceFootnote 6 may enrich our understanding of specific systems, but they are by no means necessary for giving causal explanations of natural phenomena.


