Introduction
Monitoring bird populations constitutes a vital component of biodiversity assessment and facilitates the detection of ecosystem changes on both national and international scales. In Europe, one of the most widely used monitoring frameworks is the Pan-European Common Bird Monitoring Scheme (PECBMS), which involves participation from most EU countries. The PECBMS was initiated in January 2002 as a collaborative initiative between the European Bird Census Council (EBCC) and BirdLife International (https://pecbms.info/). Its primary objective is to generate policy-relevant indicators of biodiversity trends by analysing scientific data on changes in breeding populations of common bird species across Europe. A key output of the PECBMS is the on-going provision of species population trends (https://pecbms.info/trends-and-indicators/species-trends/). The data sets have been widely utilised in various assessments, such as the Living Planet Index (https://livingplanetindex.org/), thereby enhancing our understanding of global biodiversity patterns among vertebrates. Moreover, the data support policy-making by organisations such as the European Environment Agency, European Commission, Eurostat, Forest Europe, and the Organisation for Economic Co-operation and Development, which use these data sets to report on environmental and biodiversity frameworks at both national and international levels (Brlík et al. Reference Brlík, Šilarová, Škorpilová, Alonso, Anton and Aunins2021).
Beyond its primary aim of tracking bird population trends, the PECBMS data set has also proven invaluable for ecological research. It has been used to investigate factors driving population dynamics (e.g. Burns et al. Reference Burns, Eaton, Burfield, Klvaňová, Šilarová and Staneva2021; Gregory et al. Reference Gregory, Eaton, Burfield, Grice, Ch and Klvaňová2023; Morelli et al. Reference Morelli, Benedetti and Callaghan2020; Reif et al. Reference Reif, Gamero, Hološková, Aunins, Chodkiewicz and Hristov2024), to investigate the influence of habitat characteristics and weather conditions on some bird species (e.g. Herrando et al. Reference Herrando, Brotons, Anton, Paramo, Villero and Titeux2016; Kosicki et al. Reference Kosicki, Chylarecki and Zduniak2014; Wade et al. Reference Wade, Barov, Burfield, Gregory, Norris and Vorisek2014), to assess anthropogenic impacts on migratory species (Buchan et al. Reference Buchan, Franco, Catry, Gamero, Klvaňová and Gilroy2022), and to explore mechanisms of niche divergence in closely related species (Kosicki Reference Kosicki2022, Reference Kosicki2024; Reif et al. Reference Reif, Reifová, Skoracka and Kuczyński2018). PECBMS data have also been applied to estimate the density and abundance of selected bird species at national (Chodkiewicz et al. Reference Chodkiewicz, Kuczyński, Sikora, Chylarecki, Neubauer and Ławicki2015; Hellicar and Ieronymidou Reference Hellicar and Ieronymidou2017; Norman et al. Reference Norman, Harris and Newson2012; Sudfeldt et al. Reference Sudfeldt, Dröschmeister, Grüneberg, Mitschke, Schulte and Wahl2019) and broader geographical scales (BirdLife International 2015; Keller et al. Reference Keller, Herrando, Voříšek, Franch, Kipson and Milanesi2020), informing conservation planning and the evaluation of species’ conservation status. Recent comparative work has further demonstrated the importance of integrating multiple data sources to ensure the robustness and consistency of bird population estimates across countries (Herrando et al. Reference Herrando, Fraixedas, Brotons, Martí, Staneva and Keller2024).
While PECBMS-based analysed assessments are generally regarded as reliable (Carrascal and Del Moral Reference Carrascal and Del Moral2021; Gordo Reference Gordo2018; Maggini et al. Reference Maggini, Cardinale, Favaretto, Voříšek, Spina and Maoret2021), some concerns have been raised regarding potential biases. For example, studies conducted in Spain have highlighted challenges in accurately assessing species abundance, particularly for species such as the Common Swift Apus apus and House Martin Delichon urbicum, where standard monitoring protocols (e.g. two surveys per site) may be inadequate (Gordo Reference Gordo2018). Additionally, the timing of surveys, which are typically conducted in the morning, may lead to an underestimation of species exhibiting peak activity during the evening (Kosicki et al. Reference Kosicki, Chylarecki and Zduniak2014). Furthermore, the detectability of birds is a crucial factor in wildlife surveys and has been the subject of considerable debate (Buckland et al. Reference Buckland, Anderson, Burnham, Laake and Borchers2001; Rosenstock et al. Reference Rosenstock, Anderson, Giesen, Leukering and Carter2002). Detectability is strongly influenced by the habitat occupied by a given species. To address this issue, distance sampling methods have been implemented in certain analyses (Buckland et al. Reference Buckland, Anderson, Burnham, Laake and Borchers2001).
Recognising the implications of such limitations for species conservation, particularly when abundance data are used to inform policy or management decisions, it is essential to understand how national monitoring schemes perform for species requiring particular conservation attention. One such species is the Red-backed Shrike Lanius collurio, which is listed in Annex I of the EU Birds Directive (Directive 2009/147/EC), requiring the designation of Special Protection Areas (SPAs) under the Natura 2000 network (European Commission 2009). The Common Breeding Birds Survey (MPPL; from the Polish name Monitoring Pospolitych Ptaków Lęgowych, ‘Common Breeding Bird Monitoring’) constitutes the national component of PECBMS in Poland and represents a key source of information on population trends of common breeding species. Ensuring reliable assessments of the Red-backed Shrike within this framework is therefore crucial for meeting conservation obligations and guiding effective management at both national and local scales. Although MPPL provides valuable insights into population trends, its estimates may differ from those obtained through targeted, species-specific field surveys, particularly in habitats where vegetation structure influences detectability. Understanding the nature and extent of such discrepancies is essential for improving monitoring methodologies and ensuring that conservation planning is based on robust abundance data.
The aim of this study was to assess how accurately the MPPL estimates the abundance of Red-backed Shrike at a fine spatial scale in eastern Poland. To address this aim, we compared MPPL-derived density estimates with those obtained from an independent, species-targeted field survey carried out within the same 1 × 1 km plots. We then examined discrepancies between the two approaches in relation to habitat characteristics known to be important for the ecology and distribution of the species (Lefranc Reference Lefranc2022), with particular emphasis on features likely to influence detectability. By identifying circumstances in which MPPL estimates diverge from targeted survey results, we sought to evaluate the reliability of this national monitoring scheme for an Annex I species and to determine how a generalised, multi-species protocol performs when applied to a single species with specific habitat requirements and behavioural traits. By clarifying these limitations of a widely used monitoring framework such as MPPL, our study contributes to on-going efforts to refine bird monitoring strategies and enhance their relevance for conservation practice, particularly in the context of widespread changes to agricultural landscapes that are negatively affecting bird populations across Europe (PECBMS 2024; Tryjanowski et al. Reference Tryjanowski, Hartel, Báldi, Szymański, Tobolka and Herzon2011).
Methods
Study species
The Red-backed Shrike is a small, territorial passerine bird widely distributed across Europe and western Asia. According to the PECBMS (2024), the species is undergoing a long-term decline across Europe, with a 23% reduction of population size over the past decade. In contrast, the Polish population shows moderate growth, with estimates ranging between 0.74 million and 1.1 million breeding pairs and an average density of 2.5 pairs/km² (Chodkiewicz et al. Reference Chodkiewicz, Kuczyński, Sikora, Chylarecki, Neubauer and Ławicki2015). This long-distance migrant arrives from Africa in early May, with a breeding season extending from mid-May to August (Lefranc Reference Lefranc2022). The species typically inhabits agricultural landscapes, nesting along woodland edges, in tree clusters, orchards, and currant plantations (Golawski et al. Reference Golawski, Mroz and Golawska2020). Shrikes are active throughout the day, and their frequent use of exposed perches makes them relatively easy to spot during surveys. Employing a ‘sit-and-wait’ hunting strategy, the Red-backed Shrike preys mainly on insects and typically uses elevated perches such as bushes, powerlines or fence posts (Lefranc Reference Lefranc2022; Yosef Reference Yosef, del Hoyo, Elliott and Christie2008). As such, optimal habitats are mosaics of open landscapes with shrubs and trees that allow nest establishment, and structures facilitating prey detection and capture.
Bird data collection
Fieldwork was conducted during the birds’ breeding season in 2020. Red-backed Shrike densities were assessed using two methods: a general and a targeted survey. In this study, we estimated density at the square level (hereafter referred to as ‘density’) based on 1 × 1 km survey plots. The data for the first method were obtained from MPPL from the database of the Chief Inspectorate of Environmental Protection (https://www.gov.pl/web/gios). This methodology closely aligns with the protocols established by the UK Breeding Bird Survey (Gregory and Baillie Reference Gregory and Baillie1998). A total of 1,050 randomly selected survey plots, each 1 km² in area, were distributed across a 312,000 km² area of the country. For this study, we focused on 53 plots located in eastern Poland (Figure 1). Fieldwork was conducted by trained volunteer ornithologists who systematically surveyed each plot. Each plot was visited twice: first between 15 April and 15 May, and again at least four weeks later, between 16 May and 30 June, typically during early morning hours (06h00–09h00). The mean survey duration was 85 minutes (SD = 25 minutes, range = 36–180 minutes; data pooled from two surveys). During each visit, observers walked two parallel transects, each 1 km in length and approximately 500 m apart, oriented along either a north–south or east–west axis. Birds were recorded in three distance bands: within 25 m, between 25 m and 100 m, and beyond 100 m from the transect line (Chylarecki and Jawińska Reference Chylarecki and Jawińska2007). All detections from both visits were pooled, and density estimation (see below) was based on the total effort and all observed individuals, rather than on maximum or average counts per visit.
Location of the 53 study plots (1 × 1 km each), randomly distributed across eastern Poland. The map background is based on satellite imagery from Google Earth and vector data from OpenStreetMap.

The second method involved intensive surveys of the same 53 plots (Figure 1), each visited once, conducted by the authors (AG and ZK), both of whom possess over 30 years of field experience and specialised knowledge of Red-backed Shrike ecology (e.g. Golawski and Kasprzykowski Reference Golawski and Kasprzykowski2018; Golawski et al. Reference Golawski, Mroz and Golawska2020, Reference Golawski, Mroz, Golawska, Parapura and Zduniak2023). The observers participating in the MPPL were unaware that their plots were being independently surveyed, ensuring consistency in their survey methods. These intensive surveys were conducted by the authors between 4 June and 17 July, focusing on habitats likely to support Red-backed Shrikes, such as forest edges, village peripheries, orchards, currant fields, and isolated trees or shrubs. Urban centres and large, homogeneous fields lacking nesting vegetation were excluded. To enhance detectability, we employed playback of the male’s mating call. The call was played in locations where shrikes were expected to occur (based on the observer’s experience) but had not been recorded during standard field surveys. At each such site, a 30-second call was broadcast through a loudspeaker connected to a mobile phone via Bluetooth. In areas with a continuous stretch of suitable habitat (e.g. along tree lines or forest edges), the playback was repeated approximately every 100 m. After each playback, a two-minute pause was observed to allow for a possible response. The observer took particular care to ensure that individuals approaching from outside the study area were not included in the observations. The call recording was obtained from Xeno-canto (recording no. XC478381). Surveys were carried out throughout the day, as shrikes are active from morning until evening (Golawski et al. Reference Golawski, Mroz and Golawska2020). The start time of observations at individual plots ranged from 10h23 to 18h03, with a median of 13h40. The mean survey duration was 82 minutes (SD = 25 minutes, range = 25–165 minutes), depending on the extent of suitable shrike habitats. The abundance of breeding pairs was recorded as the measure of density at the square level, as a considerable proportion of pairs already had fledglings during the survey period. Counting all individuals, as in the MPPL scheme, would therefore have substantially overestimated population size. For this reason, the number of breeding pairs was used as the standardised measure of abundance. The main differences between the two methods of estimating the number of shrikes are summarised in Table 1.
Comparison of two methods for estimating Red-backed Shrike density on 1 km2 plot size during the 2020 breeding season. MPPL = Common Breeding Birds Survey

Correlates
Building on previous research into the habitat preferences of the Red-backed Shrike (Lefranc Reference Lefranc2022), we identified several key predictors for this species. These included urban areas, arable fields, mixed crops, meadows, shrubs, and small forest patches (Figure 2; see detailed description in Supplementary material Table S1). Our analysis encompassed habitat extent, landscape metrics, and indicators of human pressure on these environments. All data were aggregated at a spatial resolution of 1 km² and reprojected to the EPSG4284 coordinate system (http://spatialreference.org/ref/epsg/4284/). Land-cover information was compiled from two primary databases. The main source was the Corine Land Cover (CLC) 2018 database, which provides raster data at a spatial resolution of 100 × 100 m, although the minimum mapping unit for land-cover classes is 25 ha. These data are based on Landsat TM remote sensing imagery and were used for land-cover types except forests, for which higher-resolution data were available. Forest areas were defined using data from the Joint Research Centre (JRC) (original download data: http://forest.jrc.ec.europa.eu/; current: https://forest.jrc.ec.europa.eu/en/past-activities/), which offers a 25-m resolution data set covering both coniferous and deciduous forests. This classification was subsequently corrected using the JRC Global Forest Cover 2020 data set (https://forobs.jrc.ec.europa.eu/GFC) to improve spatial consistency and update forest extent information. Human pressure was quantified using night light intensity, artificial light at night (ALAN), as a proxy for anthropogenic activity (Doll et al. Reference Doll, J-P and Morley2007; Small et al. Reference Small, Pozzi and Elvidge2005), (accessible at original download link: http://svs.gsfc.nasa.gov/vis/a030000/a030000/a030028/index.html; current link: https://svs.gsfc.nasa.gov/30028). All spatial data sets correspond to the period around 2020, matching the timing of the bird surveys. Additionally, using the LecoS library in QGIS (Jung Reference Jung2016), we calculated four landscape metrics for each habitat type. These included: (1) the buffer zone, defined as the area within a 100-m radius around the outer edge of each patch; (2) the core area, defined as the portion of the patch excluding the 100-m buffer. Both metrics were expressed as percentage cover within each 1 × 1 km grid cell. These metrics were calculated separately for three main habitat types, i.e. meadows, arable fields, and mixed arable fields. Additional habitat features, such as shrubs and isolated forest patches, were also extracted from CLC, but due to their small spatial extent and highly skewed distribution (often absent), only the total cover percentage within the 1 × 1 km grid was calculated for these types. Therefore, landscape metrics such as buffer zone and core area were not calculated for shrubs and isolated forests.
Mean values of predictors. Bars represent the mean values of variables describing landscape structures, and black lines indicate 95% confidence intervals. The y-axis was square-root transformed to enhance the visibility of variables with low values, such as isolated forest patches (ISL.FOR).

Data processing and analysis
We estimated bird density using line-transect distance sampling in R (package Distance; Buckland et al. Reference Buckland, Anderson, Burnham, Laake and Borchers2001; Thomas et al. Reference Thomas, Buckland, Rexstad, Laake, Strindberg and Hedley2010). Each detection was assigned to one of three distance bands from the transect: 0–25 m, 25–100 m, and 100–150 m. We truncated the data at 150 m and fitted the detection function to these binned data (cutpoints: 25 m, 100 m, and 150 m). We compared two key functions: half-normal and hazard-rate. In our data set, the half-normal model had the lower Akaike’s information criterion (AIC) (HN = 150.84; HR = 160.41) and was therefore selected for further analysis. For each 1 × 1 km plot, we set area = 1 km² and total survey effort = 4 km (two 1-km transects visited twice). No other detection covariates (e.g. time of day) were used as Red-backed Shrikes are active throughout the day, and their detectability is not strongly influenced by the time of observation. Including such covariates would therefore add unnecessary complexity without improving explanatory power or biological relevance for this species. The model returned density (individuals/km²) with standard errors. Plots with no detections were retained and reported as 0 individuals/km². In the next step, we calculated a linear regression model, where the dependent variable was the estimated density from general surveys (calculated as described above), and the explanatory variable was the density obtained from targeted surveys of the species (see Bird data collection above, ‘the second method’). We tested whether the slope of this regression line significantly differed from zero using a t-test and calculated the coefficient of determination (R²). To assess overestimation or underestimation of density, we calculated the residuals from this relationship. Negative residuals indicate a higher level of underestimation, while positive residuals suggest overestimation of the density. We then checked whether these residuals followed a normal distribution using the Shapiro–Wilk test and whether they differed significantly from zero using t-test. After confirming these assumptions, we analysed the residuals using a Generalised Linear Model (GLM) (Gaussian error, identity link) to identify which environmental factors might influence the degree of underestimation or overestimation. As predictors we used: built-up area, meadows, mixed crops, shrubs, three buffer variables (arable, meadows, mixed crops), small forest patches, and ALAN. We included linear terms for all predictors, and quadratic term (x²) for buffer variables potential non-linear effects. Variables were mean-centred prior to squaring to reduce multicollinearity. The full candidate model was:
 $$ {residual}_i={\beta}_0+\sum \limits_{k=1}^K{\beta}_k{X}_{k,i}+\sum \limits_{b\in B}{\gamma}_b{C}_{b,i}^2+{\varepsilon}_i,\hskip0.48em {\varepsilon}_i\sim N\;\left(0,{\varepsilon}^2\right) $$
where i = index of the plot (sample), X
k,i = linear environmental covariates (e.g. built-up, meadows, mixed crops, shrubs, small forest patches, ALAN), B = set of buffer variables, Cb,I = centred variable (value minus the mean); in the model we use only the squared term, C2
b,I = to capture simple curvature (U- or inverted-U shape), β = intercept, βk, γb = effect coefficient,
 $ \hskip0.48em {\varepsilon}_i $
= error term. Model diagnostics are provided in Figure S2).
We ranked all model subsets by Akaike’s information criterion corrected for small sample sizes (AICc) (MuMIn) and selected the model with the lowest AICc (Akaike weights are reported). We checked multicollinearity using the variance inflation factor (VIF) (threshold <5) and pairwise correlations (|r| <0.7). As a measure of fit, we report pseudo-R² = 1 (residual deviance/null deviance).
To construct all possible combinations of predictors, we used MuMIn::dredge based on the full GLM. The error structure and link were fixed (Gaussian, identity), and the intercept was retained. We did not include interactions. We enforced a simple hierarchy rule: a quadratic buffer term (x²) could enter the model only together with its linear parent (x). With this rule the procedure produced 511 candidate models. We then ranked the models by AICc and selected the model with the lowest AICc and highest Akaike weights.
Results
Densities from MPPL and targeted surveys
The mean density of Red-backed Shrike obtained from targeted surveys was 3.9 breeding pairs/km² (95% CI: 3.08–4.72; range: 0–13), whereas the mean estimated density based on MPPL data was 2.1 individuals/km² (95% CI: 1.42–2.82; range: 0–11.57). Although the paired t-test revealed a significant difference in densities between the targeted survey and MPPL estimates (t = 5.26, df = 52, P <0.0001), we found a linear relationship between these two kinds of abundance estimates (β ± SE = 0.51±0.09, t = 5.43, P <0.001, R² = 0.36) (Figure 3).
Relationships between targeted and Common Breeding Birds Survey (MPPL) estimated Red-backed Shrike density.

Residuals from this linear regression ranged from -4.22 to 4.78, did not differ significantly from zero (t = 0.0003, P = 0.999), and followed a normal distribution (W = 0.97, P = 0.20). Negative residuals indicate cases where the MPPL-estimated density was lower than that from targeted surveys (but the degree of underestimation decreases as residuals approach zero), while positive residuals reflect cases where the MPPL-estimated density exceeds the targeted survey density.
Expected and targeted survey density
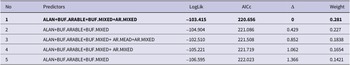
Out of 511 candidate GLMs (all-subsets derived from the full model), the top-ranked model (based on AICc) included ALAN, the buffer of arable fields, the buffer of mixed crops, and area of mixed crops (Table 2). The pseudo-R² of the most parsimonious was 0.264. Two predictors were significant: buffer of arable fields (β = −0.0829 ± 0.0311 SE, t = −2.665, P = 0.010; Figure 4A) and buffer of mixed crops (β = −0.0327 ± 0.0121 SE, t = −2.709, P = 0.009; Figure 4B). ALAN (β = −0.0978 ± 0.0531 SE, t = −1.840, P = 0.072) and mixed crops (β = 0.0205 ± 0.0123 SE, t = 1.666, P = 0.102) were not significant. Thus, this analysis indicates that as the proportion of buffer zones for arable fields and mixed crops in grid cells increases, MPPL-based estimates tend to increasingly underestimate Red-backed Shrike densities relative to those obtained from the targeted surveys.
Summary of candidate Generalised Linear Models (GLMs). The models vary in their inclusion of environmental predictors, i.e. urban areas, meadows, mixed crops, shrubs, buffer zones around arable fields, meadows, and mixed crops, forest islands, and artificial light at night (ALAN). Models are ranked by Akaike’s information criterion corrected for small sample sizes (AICc), with associated log-likelihood (LogLik), AICc differences (ΔAICc), and Akaike weights (weight). The most parsimonious model is highlighted in bold
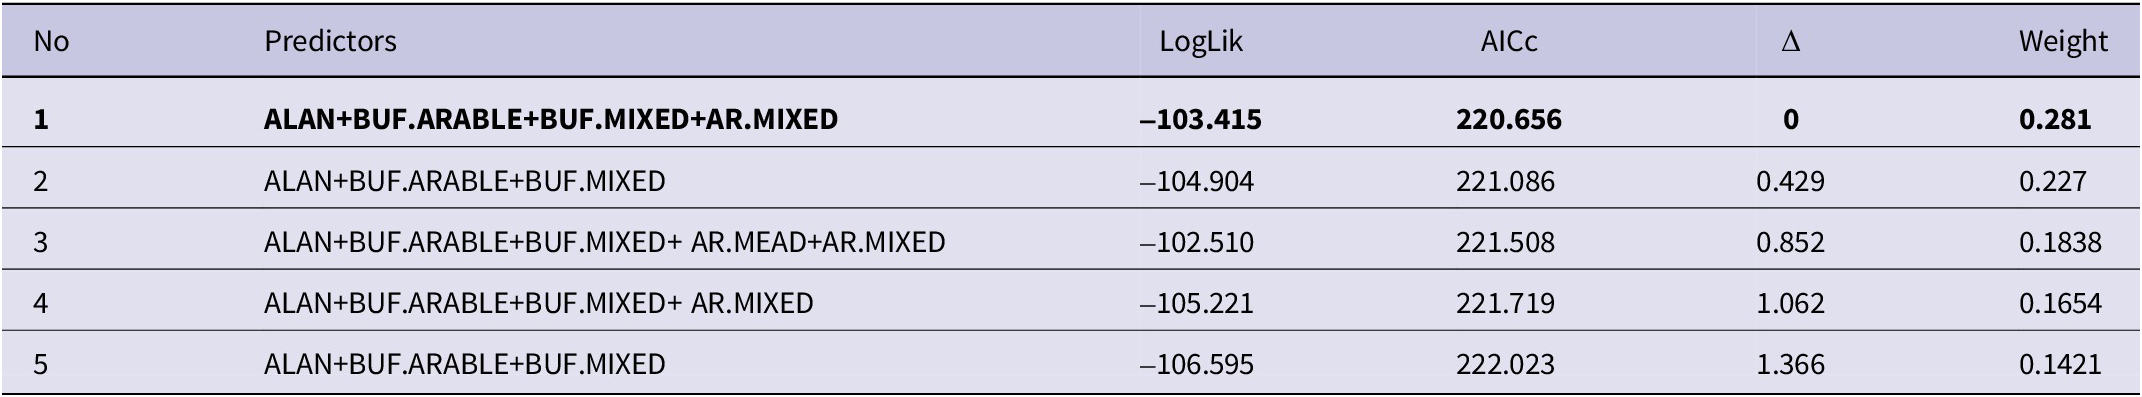
Relationship between the residual difference in Red-backed Shrike density between targeted and Common Breeding Birds Survey (MPPL)-monitoring estimated density and the share of buffer zones within 1 × 1 km cells: (A) arable fields and (B) mixed crops. Solid lines show the fitted partial effect from the top-ranked Gaussian Generalised Linear Model (GLM), with shaded ribbons indicating 95% confidence intervals.

Discussion
Our study revealed that density estimates of the Red-backed Shrike obtained from MPPL differed from targeted field surveys. While MPPL estimates were systematically lower than targeted survey densities, a significant linear relationship was identified between the two data sets, suggesting that MPPL data provide a reasonable approximation of Red-backed Shrike densities, sufficient to compare density indices between different surfaces in wide spatial domains.
Among the tested habitat variables, only buffer zones around arable fields, and buffer zones around mixed crops showed significant relationships with discrepancies in density estimates. Importantly, such discrepancies are expected because the two approaches employ fundamentally different protocols: MPPL uses standardised, multispecies transects optimised for broad-scale inference, whereas our targeted surveys were explicitly species-specific (habitat-focused, with playback and later-season timing), inherently yielding higher detectability for shrikes. Hence, the observed differences reflect methodological design rather than a flaw of MPPL. The discrepancies observed were linked to specific habitat features, especially the structure and coverage of buffer zones within grid cells.
A further issue also requires consideration. The MPPL method expresses density as the number of individuals, whereas in the targeted field survey it was expressed as the number of pairs. MPPL data may therefore partly include both sexes forming pairs. To assess the magnitude of this effect, we summarised national MPPL data from 2020 (788 survey plots): during the first visit, 113 males and 24 females (plus 68 of undetermined sex) were recorded, and during the second, 437 males and 95 females (plus 316 unsexed). Among sexed individuals, males constituted 82.5% and 82.1% during the first and second visits, respectively. These proportions indicate that the difference between counts of individuals and pairs is not large, with MPPL likely overestimating pair-based densities by less than 19%. Accordingly, the mean MPPL value of 2.1 individuals/km² would correspond to approximately 1.8 pairs/km².
We speculate that the differences in bird density estimates derived from the two counting methods are due to the diverse structure of buffer zones, which include shrubs, isolated bushes, and trees. Such buffer zones are classified as ecotone zones, characterised by scattered shrub and tree vegetation, which may constitute the most important habitats for shrikes at the landscape scale (Brambilla et al. Reference Brambilla, Casale, Valentina, Crovetto, Falco and Negri2009; Ceresa et al. Reference Ceresa, Bogliani, Pedrini and Brambilla2012; Polak Reference Polak2012). Detecting shrikes within the strictly defined MPPL methodology, where observers follow transects, is particularly challenging in such areas due to visual obstructions created by scattered bushes and trees. This pattern aligns with a mechanism where vegetation structure simultaneously provides resources and decreases detectability.
The moderate pseudo-R² value in the final GLM model suggests that, while habitat metrics explain some variability in density estimation errors, other factors – such as observer experience or variability in shrike detectability across daily or seasonal cycles – may also play a significant role. Similar challenges have been reported in studies of other bird species, where time of day (e.g. Kosicki et al. Reference Kosicki, Chylarecki and Zduniak2014) and observer turnover (Vallecillo et al. Reference Vallecillo, Gauthier-Clerc, Guillemain, Vittecoq, Vandewalle and Roche2021) affected data reliability. Observers participating in the MPPL are trained and evaluated for their species identification skills; however, differences in experience and familiarity with specific habitats may influence detection rates. In contrast, targeted surveys conducted by highly specialised observers, who employed vocal stimulation to increase detectability, likely achieved higher detection success. Nevertheless, even these focused surveys could not detect all nesting pairs (see Tryjanowski et al. Reference Tryjanowski, Hromada, Antczak, Grzybek, Kuźniak and Lorek2003), highlighting the inherent challenges of achieving complete detection in avian monitoring programmes.
The timing of the MPPL surveys also impacts bird detectability. The standards for the first survey date (15 April to 15 May) mean that many surveyed fields are inspected before the shrikes arrive. Although some individuals may arrive by late April, substantial numbers typically appear only after 10 May (Golawski et al. Reference Golawski, Mroz and Golawska2020). The second MPPL surveys occur between 15 May and 30 June, but guidelines advise against scheduling them too late due to reduced activity in many species. Red-backed shrikes in east-central Poland start breeding (laying their first egg) on average on 1 June, resulting in low detection rates for females in June (Golawski et al. Reference Golawski, Mroz and Golawska2020, Reference Golawski, Mroz, Golawska, Parapura and Zduniak2023; Tryjanowski et al. Reference Tryjanowski, Hromada, Antczak, Grzybek, Kuźniak and Lorek2003). Females become more active only during the second week of the nestlings’ life, which typically falls after 20 June. During incubation and the first week of the nestlings’ life, as a rule, only the feeding male is generally visible (Golawski et al. Reference Golawski, Mroz, Golawska, Parapura and Zduniak2023), which significantly reduces the detection rate of the species (see also Morelli et al. Reference Morelli, Mroz, Pruscini, Santolini, Golawski and Tryjanowski2016, for sex- and stage-related differences in hunting activity). This temporal mismatch between standardised monitoring windows and the phenology of target species may result in systematic underestimations, especially for taxa with sex-biased detectability during breeding. Our targeted observations were most intense at the end of June and continued until 17 July, when most pairs had fledged their young but remained within their breeding territories. During this period, birds were active, bringing food to fledglings, the begging calls of young were audible, and shrikes typically displayed alarm behaviour from considerable distances (Tryjanowski and Golawski Reference Tryjanowski and Golawski2004; Tryjanowski et al. Reference Tryjanowski, Hromada, Antczak, Grzybek, Kuźniak and Lorek2003). Together, these phenological considerations explain why species-specific protocols timed to fledgling care can outperform early season multispecies windows for shrike detection.
To quantify how much variance our two-stage approach explains (1. deriving the response and 2. modelling it), we accounted for sequential variance partitioning. First, the regression MPPL ~ targeted gives R-squared = 0.36, leaving 64% unexplained. Second, the GLM fitted to the residuals had pseudo-R² = 0.26. On the original scale, this adds 0.64 × 0.26 = 0.1664 to the explained share. Therefore, the total explained variance is 0.36 + 0.1664 = 0.526, meaning that about 47% remains unexplained, likely due to unmeasured factors such as time of day, playback details, fine-scale habitat, detection heterogeneity, and sampling noise. This highlights the complexity of factors influencing detectability, including microhabitat structure, temporal variation, and observer effects (Buckland et al. Reference Buckland, Anderson, Burnham, Laake and Borchers2001; Rosenstock et al. Reference Rosenstock, Anderson, Giesen, Leukering and Carter2002). In light of this, enhancing monitoring schemes through integration with habitat-specific data, remote sensing technologies or adaptive timing of surveys could significantly improve accuracy for conservation-relevant metrics. Nevertheless, while MPPL data may not be well-suited for estimating absolute densities at fine spatial scales, they remain an invaluable tool for deriving population indices and tracking long-term trends across broad geographical regions (Gregory et al. Reference Gregory, Vorisek, Noble, Van Strien, Klvaňová and Eaton2008; Herrando et al. Reference Herrando, Brotons, Anton, Paramo, Villero and Titeux2016). This is precisely the mandate of MPPL, which focuses on broad-scale, multispecies indicators, and our findings should be interpreted as a complement to that remit rather than as a criticism. Their application in large-scale biodiversity monitoring provides critical insights into population dynamics, enabling evidence-based conservation strategies and policy-making.
In conclusion, our study highlights discrepancies between Red-backed Shrike density estimates from large-scale bird monitoring and targeted field surveys. MPPL estimates were generally lower but moderately correlated with target surveys. Habitat characteristics identified as significant factors influencing detection accuracy included buffer zones around arable fields and mixed crops. These habitats likely provide critical resources for shrikes, such as shrubs or clumps of vegetation, while simultaneously hindering their detection. Timing of surveys and species-specific breeding behaviours further contribute to variability. These findings emphasise the limitations of generalised monitoring protocols like MPPL, which are designed primarily for large-scale comparisons and multispecies assessments, rather than precise density estimation at fine spatial scale. Caution should therefore be exercised when applying such data to detailed ecological studies of individual taxa, such as the Red-backed Shrike. Future efforts to improve monitoring accuracy should consider species-specific detectability patterns and optimise survey timing to enhance the value of national schemes for conservation-oriented decision-making. Nevertheless, any refinement of survey protocols must balance improved accuracy for individual species with the practical constraints inherent in large-scale, multispecies monitoring. For example, while later surveys could enhance detectability of the Red-backed Shrike, they might reduce detectability of early breeding species. A feasible solution would be to implement complementary, species-focused checks on a subset of plots (or in priority habitats) within the existing framework, thereby improving inference for focal taxa without compromising the multispecies scope of MPPL.
Supplementary material
The supplementary material for this article can be found at http://doi.org/10.1017/S0959270925100373.
Acknowledgements
We would like to thank all the observers who took part in the field surveys, as well as everyone who contributed to the data analysis. The MPPL programme is carried out in Poland by volunteers cooperating with the Polish Society for the Protection of Birds (OTOP BirdLife Poland). It is commissioned by the Chief Inspectorate for Environmental Protection and funded by government institutions. We thank Sara Wild for English language editing. We are also grateful to the anonymous reviewers for their insightful comments and constructive suggestions, which greatly improved this paper. The research was supported by the University of Siedlce, Poland. Author contributions: conceptualisation: AG, ZK, JK; methodology: AG, ZK; formal analysis: JK; investigation: AG, ZK; monitoring data: TC, ŁW; writing – original draft preparation: all authors; writing – review and editing: all authors.