1. Introduction to the Problem
At least since Locke (Reference Locke1689, Book 2, Chapter viii),Footnote 1 color scientists and philosophers have been inclined to deny any objective reality to the familiar ontology of perceivable colors, on grounds that physical science has revealed to us that material objects have no qualitative features at their surfaces that genuinely resemble the qualitative features of our subjective color experiences. Objective colors are therefore dismissed as being, at most, “a power in an object to produce in us an experience with a certain qualitative character.” Accordingly, colors proper are often demoted from being ‘primary properties’ (i.e., objective properties of external physical objects) to the lesser status of being merely ‘secondary properties’ (i.e., properties of our subjective experiences only).
To be sure, we are not logically forced to this eliminative conclusion by the failure of the first-order resemblances cited. A possible alternative is simply to identify each of the familiar external, commonsense colors with whatever “power within external objects” it is that tends to produce the relevant internal sensation. More specifically, we might try to identify each external color with a specific electromagnetic reflectance profile had by any object that displays that color. The objective reality of colors would then emerge as no more problematic than is the objective reality of the temperature of a gas (which is identical to the mean kinetic energy of its molecules), or of the pitch of a sound (which is identical to the dominant oscillatory frequency of an atmospheric compression wave), or of the sourness of a spoonful of lemon juice (which is identical with the relative concentration of hydrogen ions in that liquid). These parallel properties also fail the ‘first-order resemblance’ test imposed by Locke and other Early Modern thinkers. Nonetheless, their successful reduction to objective properties of material objects is an accomplished fact, both of science and of settled history. Locke's criterion for objective reality—a first-order resemblance to the qualities of our sensations—was simply ill conceived.
On the more modern reductive approach displayed in these examples, color may turn out to be, by the standards of uninformed common sense, a somewhat surprising sort of feature, namely, a profile of reflectance efficiencies across the visible part of the electromagnetic spectrum. But this is no more surprising than any of the other identities just cited. And no more surprising, perhaps, than the identification of light itself with electromagnetic waves. Such identities may surprise the scientifically uninformed, but they leave the objective reality of light, temperature, pitch, and sourness entirely intact.
Unfortunately, this happy (reductive) accommodation would seem to be denied us in the case of colors in particular. For, it is often argued, there is no unique electromagnetic reflectance profile that corresponds to, and might thus be a candidate for identification with, each (or, indeed, any) of the familiar colors. On the contrary, to each of the familiar colors there corresponds an apparently unprincipled variety of decidedly different reflectance profiles. The scattered class of such diverse profiles, for each ‘objective’ color, is called the class of metamers for that color, and they are indeed diverse, as the four profiles in Figure 1 illustrate.
Figure 1.

Four distinct material objects, each boasting one of the four reflectance profiles here portrayed, will appear identically and indistinguishably yellow to a normal human observer under normal illumination (e.g., in broad daylight). And these four profiles are but a small sample of the wide range of quite distinct reflectance profiles that all have the same subjective effect on the human visual system. The fact is, our rather crude resources for processing chromatic information—namely, the three types of wavelength-sensitive cone cells and the three types of ‘color-opponency’ cells to which they ultimately project—are simply inadequate to distinguish between these metamers. Any object boasting any one of them will look to be a qualitatively uniform yellow, at least under normal illumination.
These examples concern the color yellow, but a similar diversity of same-looking metamers attends every other color as well. If one had hopes for a smooth reduction of each of the commonsense colors to a uniquely corresponding reflectance profile, those hopes are here frustrated: first, by a real diversity of reflectance profiles corresponding to each visually distinguishable color; and second, by our apparent inability to characterize what unifies the relevant class of diverse reflectance profiles, appropriate to each visually distinguishable color, independently of appealing to the qualitative character of the visual sensations they happen to produce in the idiosyncratic visual system of the human brain. If that is the only way in which we can specify what unites the class of metamers specific to any color, then either we must resign ourselves to a deflationary relational reconstrual (Cohen Reference Cohen2004) of what common sense plainly takes to be monadic properties of material objects, or we must resign ourselves to the elimination of objective colors entirely, as Hardin (Reference Hardin1993, 300, n. 2), coherently enough, recommends.
2. Reformulating the Problem
That the apparently unprincipled diversity of metamers poses a genuine problem for a reductive account of objective colors can be seen from a second perspective, one of central importance for understanding how the brain portrays the external world. A promising general approach to understanding how the brain—or any of its various subsystems—represents the external world posits the brain's development, through learning, of a variety of (often high-dimensional) maps of the objective similarity-structure of this, that, or the other objective feature-domain. Through extended experience with the relevant objective feature-domain, the relevant part of the brain can construct an internal map of that domain—of the range of possible faces, the range of possible voices, the range of possible reaching motions, the range of possible colors, and so forth. Such internal maps represent the lasting or fixed structure of each external feature-domain, and they constitute the brain's general knowledge of the world's objective structure, that is, of the entire range of possible features that the world might display at any given time and place.
Once these conceptual resources are in place, the ongoing activity of the brain's various sensory systems will produce fleeting activations at specific locations within those acquired background maps, activations that code or index where, in the space of background possibilities comprehended by the map, the creature's current objective situation is located. For example, I am now looking at my wife's face; I am listening to my wife's voice; she is reaching for a coffee mug; and that coffee mug is white. In sum, I have a background conceptual framework—or, rather, an interconnected system of such frameworks—and my sensory systems keep me updated on which of the great many possibilities comprehended by those frameworks are actualities here and now.
But the informational quality of such sensory indexings is profoundly dependent on the antecedent representational virtues of the background framework in which they fleetingly occur. The basic virtue of such background maps—as with any map—is a structural homomorphism between the map-as-a-whole, on the one hand, and the entire feature-domain that it attempts to portray, on the other. The family of proximity relations that configure the many map elements of the brain's internal mapFootnote 2 must have a relevant homomorphism with the family of similarity relations that configure the many landmark features within the domain-to-be-portrayed. Such homomorphisms or second-order resemblances, on this view, are the essence of the brain's representational achievements. One might call this account “domain-portrayal semantics,” to contrast it with such familiar doctrines as indicator semantics or causal covariation semantics.
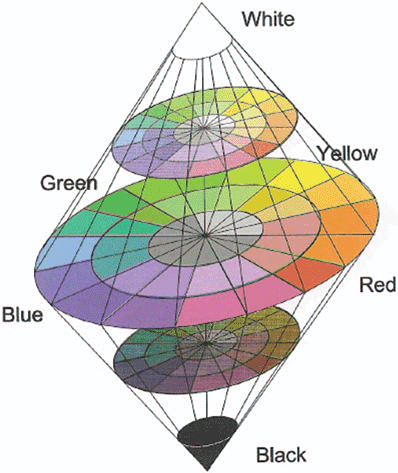
I will not pause, in this essay, to detail the many virtues of this unified approach to how the brain represents the world's general or background categorical structure, and how it represents the world's local configuration here and now.Footnote 3 I sketch it here because it provides the background for a powerful contemporary objection to the reality of external colors in particular. “How,” it may be asked, “does the peculiar and well-defined three-dimensional structure of the human phenomenological color space (see the spindle-shaped solid in Figure 2) map onto the objective space of possible electromagnetic reflectance profiles displayed by material objects? What is the internal structure of that objective target feature-domain in virtue of which the internal structure of our phenomenological color spindle constitutes an accurate map of that target domain?”
Figure 2.

The objector's questions here are, of course, semirhetorical. The point is to emphasize the presumed fact that there is no objective structure that nicely configures the range of possible reflectance profiles displayed by material objects. Collectively, they form a noisy and unprincipled scatter of possibilities. At the very least, if there is some structure within that range of possibilities, it fails to answer in any way to the very specific and demanding structure displayed in our phenomenological color spindle. Objective colors, one might therefore conclude, are a “grand illusion.” The objective reality, concerning the surfaces of physical objects, is distinctly and importantly different from the naïve assumptions of common sense and from the crude and misleading deliverances of our native sensory equipment (see Thompson, Palacios, and Varela Reference Thompson, Palacios and Varela1992, 16; Hardin Reference Hardin1993, 300, n. 2).
This is, at least potentially, a very powerful argument against any commonsense view of colors as objective features of material objects. It appeals to the correct account of how objective feature-domains get represented in and by a brain, and it points to an apparently massive failure of the required second-order or structural representation in the specific case at issue. The unreality of objective colors is the presumptive consequence.
Nonetheless, I shall presume to resist this argument, because I think it rests on a false premise. Despite a negative first impression, there is a way to construe the initially opaque space of possible reflectance profiles so that its structural homomorphism with human phenomenological space becomes immediately apparent. Accordingly, our color space does map an objective reality after all, I shall argue, and thus the argument against color realism evaporates.
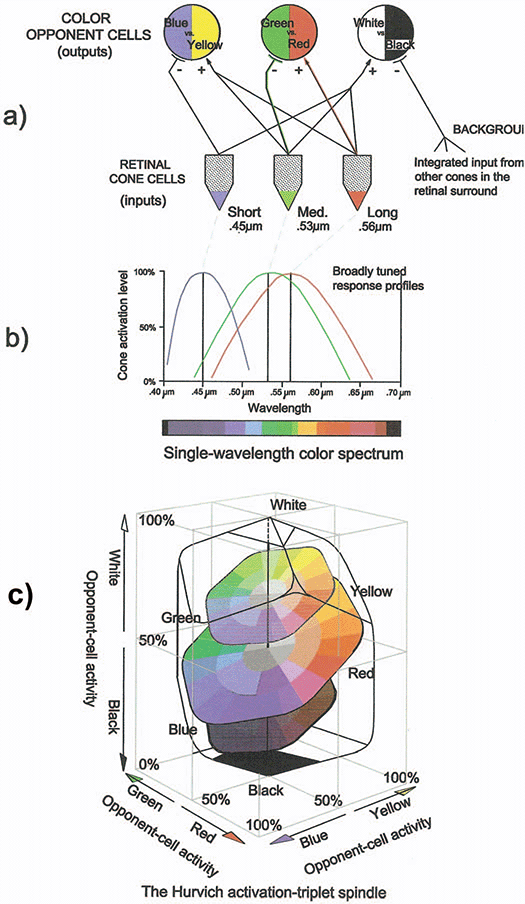
We understand one-half of this ‘mapping conundrum’—namely, our phenomenological color space—quite well, both empirically and theoretically. The now-familiar Hurvich-Jameson opponent-process, neural-network model of human color coding provides a compelling reconstruction of the empirical details of the spindle-shaped color solid of Figure 2. Figure 3a portrays the connectivity of that network, and Figure 3b portrays the wavelength sensitivity profiles of the three types of input cones. If one calculates the full range of possible activation patterns across the three types of second-layer color-coding cells, given the details of the network's connectivity, that color-coding space turns out to have the shape portrayed in Figure 3c. Evidently, it has the same dimensionality, shape, and representational organization of the empirical color spindle, wherein lies its claim to explain the organization of our phenomenological color space (for the details, see Churchland [Reference Churchland2005]). This half of our problem—namely, the nature and ground of our internal map—is stable and more or less settled. It is the nature of the external reality being mapped that needs to be importantly reconceived.
Figure 3.

3. Reconfiguring the Space of Possible-Reflectance-Profiles
The conventional way of representing any given reflectance profile, located within the narrow window of the visible spectrum (see Figure 4a), positively hides an important feature of the range of possibilities therein comprehended. Perhaps the first hint of an alternative mode of representing those possibilities arises from the fact that the phenomenological color that corresponds to any narrowly monochromatic stimulus varies continuously across the visible spectrum, but it tends toward the same color—as it happens, a sort of deep purple/magenta—at each of the two opposite extremes: .40 μm at the extreme left and .70 μm at the extreme right. It doesn't quite get there in either case, for no single wavelength of light will produce a sensation in the purple/magenta range. To get that (strictly nonspectral) range of colors, you need simultaneous retinal stimulations at two places in the visible spectrum, toward its left and right extremes, respectively. But purple/magenta remains the missing color toward which each extreme tends. (Everyone since Newton has acquiesced in his constructing a continuous ‘color wheel’ in which the nonspectral purples are interposed to fill in the ‘similarity gap’ left open by the full range of single-wavelength stimuli.Footnote 4) One's sense of rightful symmetry might therefore suggest that—as no more than an idle exercise, perhaps—one should pick up the planar figure in 4a and roll it into a cylinder so that its right-most vertical edge makes a snug contact with its left-most vertical edge, as in Figure 4b. This converts the original planar space into a space that has no boundaries in the horizontal direction. It has boundaries only at the top and bottom of the space.
Figure 4.

This trick turns the original reflectance profile itself, whatever its idiosyncratic ups and downs, into a wraparound configuration that admits of an optimal approximation by a suitable planar cut through the now-cylindrical space. The locus of any such planar cut through the cylinder will always be an ellipse of some eccentricity or other (a circle in the limiting case of a planar cut that is orthogonal to the cylinder), as portrayed in Figure 5b.
Figure 5.

The peculiar ellipse produced by a specific cut will be said to be an optimal—or, as I shall say henceforth, a canonical—approximation of the original or target reflectance profile when it meets the following two defining conditions:
1. The altitude of the ellipse must be such that the total area A above the canonical ellipse, but below the several upper reaches of the target reflectance profile, is equal to the total area B beneath the canonical ellipse, but above the several lower reaches of the target reflectance profile. (This condition guarantees that the total area under the target reflectance profile equals the total area under the approximating ellipse.)
2. The angle by which the ellipse is tilted away from the horizontal plane, and the rotational or compass heading positions of its upper extreme, must be such as to minimize the magnitude of the two areas A and B. (This condition guarantees that the approximating ellipse follows the gross shape of the target reflectance profile, at least to the degree possible.)
A suitably situated, tilted, and rotated ellipse that meets these optimizing conditions, for a given reflectance profile, will be said to be the canonical approximation of that profile. Note that an indefinite variety of distinct reflectance profiles can share the very same ellipse as their canonical approximation. That clustering population, I shall propose, constitutes the class of metamers for whatever ‘seen color’ is produced by an object with a reflectance profile that displays their shared canonical approximation.
Equally important, for each and every individual reflectance profile, however jagged, there is a unique canonical approximation. (This is a consequence of sheer geometry and of the definition provided above.) Note also that the canonical approximation for a given profile is an objective fact about that profile and about the material object that possesses that profile. Its specification makes no reference to the human visual system nor to the nature of its phenomenological responses to anything. The canonical approximation for the reflectance profile of a given material thing is an objective, mind-independent feature of that material thing. We can safely be realists about whether a given reflectance profile has a specified ellipse as its canonical approximation (for short, its “CA-ellipse”), just as we can safely be realists about the reflectance profile thereby approximated.
4. How the Human Visual System Tracks CA-Ellipses
Having identified such an objective, mind-independent feature of material objects, we might be tempted, straightaway, to identify any objective color with the canonical approximation of the relevant material object's reflectance profile. But this is emphatically not my purpose. As will emerge, my aim is the more narrowly focused aim of identifying colors proper with the original, fine-grained reflectance profiles themselves, and not with their canonical approximations. But more of that in a moment. For the present, I wish to point out that the changing activities of the human visual system—as explored experimentally by generations of psychologists since Munsell, and as portrayed in the familiar Hurvich-Jameson network's (Hurvich Reference Hurvich1981) theoretical reconstruction of our phenomenological color space (once again, see Figure 3c)—track the canonical approximations of the sundry reflectance profiles of various material objects very effectively indeed. Let me illustrate, and let us begin by simply examining the global structure of a new space: the entire space of possible CA-ellipses.
The first thing to appreciate is that the space of possible CA-ellipses has three dimensions of variation: (1) the vertical position or altitude of the given ellipse's center point within the reflectance-profile cylinder of Figure 6a; (2) the degree to which that ellipse is tilted away from being perfectly horizontal; and (3) the rotational position, around the cylinder, of that ellipse's highest point. This three-space is clearly finite, and it boasts the global shape portrayed in Figure 6b.
Figure 6.

Note well its spindle-like or football-like configuration. The horizontal dimension (orthogonal distance away from the vertical central axis) shrinks sharply to zero as the extreme top and bottom of the space are approached. This reflects the fact that any CA-ellipse in Figure 6a will be progressively ‘forced’ into an increasingly horizontal position as its altitude approaches the upper or lower extremes of the rolled-up reflectance-profile space. Its ‘tilt’ must fall to zero as its altitude is forced ever closer to the ceiling or the floor of that cylinder. Accordingly, the horizontal dimension of the CA-ellipse space, which represents that tilt, must also tend to zero at both the top and bottom of that space's vertical axis.
That tilt, recall, ultimately represents the degree to which an object's reflectance profile strongly favors some particular region of wavelengths over all the other wavelengths in the spectral window .40–.70 μm. And that dimension of variation corresponds very closely indeed to the dimension of color saturation displayed in the original phenomenological color solid of Figure 2. That dimension, of course, also shrinks to zero at the top and bottom extremes of that original space, wherein reside the hueless maximally bright white and the hueless maximally dark black, respectively.
To continue, the vertical dimension of the CA-ellipse space represents the altitude of a given ellipse's center point along the central axis of the reflectance-profile cylinder, which altitude ultimately represents the total area under the CA-ellipse. That is, it represents the total energy of both the original reflectance profile itself and its CA-ellipse (these, recall, are always the same). And that dimension of variation corresponds very closely indeed to the dimension of color brightness and darkness displayed in the original phenomenological color solid of Figure 2. That dimension bottoms out at maximal black and proceeds upward through its central axis to progressively lighter shades of gray, until it tops out at maximal white. In between those dark/light extremes, and away from the central axis toward the phenomenological space's outer surface, the various hues proceed from dark and weakly saturated versions of each (i.e., muddy versions), through maximally vivid or saturated versions at the equator, through progressively lighter and more weakly saturated versions of each (i.e., pastel versions) as we move up the color spindle. Here again, we confront another salient dimension of variation within our phenomenological space that corresponds very closely, this time, to the vertical dimension of the CA-ellipse space of Figure 6b. Brightness, evidently, is the objective feature therein represented.
Finally, there remains the dimension of angular position around the central axis of the CA-ellipse space. This dimension of variation reflects the angular position of the objective high point of the given CA-ellipse in the rolled-up reflectance-profile space of Figure 5b, which corresponds, in turn, to the seen hue within the phenomenological color solid of Figure 2. Evidently, a physical object's hue is the objective feature therein represented.
The CA-ellipse space (Figure 6b), let us remind ourselves, contains only points. (It is the rolled-up reflectance-profile space that contains the jagged profiles themselves and the wobbling ellipses that variously approximate them.) But that CA-ellipse space displays, immediately, exactly three dimensions, each one of which corresponds to a salient dimension of our antecedently appreciated subjective phenomenological color space, which also has three dimensions. Moreover, each of these two spaces displays the same global shape: something close to a spindle or a football. Additionally, both spaces code the brightest objects at the upper tip of their spindles and the darkest objects at the very bottom. Finally, both spaces code for the very same hues in their corresponding equatorial positions, in the same sequence as we proceed around that equator. Altogether, the internal structure of our subjective phenomenological color space provides an unexpectedly accurate map of the internal structure of the entirely objective CA-ellipse space.
Exactly how accurate is it? Topographically speaking, it is the answer to a color realist's prayer. It has three dimensions, exactly two of which present themselves in polar coordinates. It has the same global shape. And apparently it has all the same betweenness relations. But how accurate is it metrically?
It is very good, but not perfect. First, our phenomenological map is metrically deformed, somewhat, in the green/yellow/orange/red region, where the human L-cone sensitivity curve and the M-cone sensitivity curve substantially overlap each other (see again Figure 3b). This idiosyncratic feature of the human visual system for detecting color samenesses and differences makes us slightly hyperacute in that region. Because of this overlap, our color-processing system is here more sensitive to small changes in the dominant incident wavelength than it is to wavelength changes elsewhere in the optical window: in the short-wavelength or blue region, for example. The result is that the system counts smallish wavelength changes in the green through red region as equal in magnitude to somewhat larger increments of wavelength change elsewhere. You can see this metrical deformation directly by looking at the familiar rainbow-like color bars underneath Figures 1a–1d. Those bars mark off equal increments of wavelength, but the ‘seen colors’ that correspond to them change only slowly in the blue region to the left, but rather more quickly in the green to red region toward the right.
Metrical deformations of some kind are a familiar feature of real-world maps. Think of the early-modern maritime maps made of the Americas. These were fairly accurate in the vertical direction, since the map-making ship's latitude was easily reckoned by the maximum nighttime altitude, above the horizon, of familiar stars. But they were notably inaccurate in their horizontal dimension, since the earliest expeditions had no accurate clocks, and thus no surefire way of determining their east-west or longitude position as they made charts of their target coastlines. The western coast of North America, for example, was occasionally misportrayed as tilting almost 45° to the left of its actual profile, all the way up to Vancouver Island. Their inaccuracies aside, those maps were still maps. A more exaggerated example of metrical deformation is that displayed in any Mercator projection of the earth's surface, such as still grace the walls of every grade school classroom in America. As one approaches the northern and southern extremes of such maps, their metrical (mis)representation of east-west distances grows to absurd proportions. These gross metrical failings notwithstanding, the Mercator projection of the earth's surface remains a paradigm example of a map, and a very useful one at that. Overall, and metrically speaking, our color map is much more accurate than a Mercator map of the earth.
Second, and as is to be expected, our internal phenomenological map shows a nontrivial metrical deformation—this time in the vertical or brightness dimension—in the areas toward the extreme left and the extreme right of the optical window portrayed in Figure 1, for this is where the absolute sensitivity of our S-cones and our L-cones falls to zero.Footnote 5 As with measuring instruments generally, the accuracy of our color-processing system plunges swiftly as one tracks its performance at the extreme limits of its proprietary range of sensitivity. Specifically, reflectance profiles with a substantial but isolated spike hard against either end of the .40–.70 μm window will get (mis)represented as being essentially hueless and as being much darker than they objectively are. In these narrow regions the visual system fails to track accurately the objective tilt and altitude of a profile's CA-ellipse, at least if the relevant ellipse owes its proprietary configuration to a large reflectance spike confined to that insensitive region. Such residual representational failures are inevitable. They represent genuine, if minor, defects in the human visual system for representing objective color, but they do not represent any defect in the claim that the human visual system does represent objective CA-ellipses. For it remains true that, these minor defects aside, the phenomenological space in which our visual system codes its measurements plainly does constitute a recognizable map of the space of CA-ellipses for objective reflectance profiles.
Moreover, and as if to make amends for its representational failures at, or very close to, the atypical .40–.70 μm boundary of the rolled-up reflectance-profile space of Figure 4b, the human visual system does indeed make effective discriminations of the actual configuration of CA-ellipses whose high point lies anywhere close to that problematic boundary if, but only if, the reflectance profiles thereby approximated possess the bulk of their energies at two distinct wavelength spikes at some distance on either side of that discriminational ‘dead point’. In fact, it is precisely such two-headed profiles that get coded, by the human visual system, with the familiar (but appropriately nonspectral) purples!
This idiosyncratic feature of human color coding has been familiar to color scientists for many years (see again Hardin Reference Hardin1988, 115, Figure III-1). The CA-ellipse story of what it is that our visual system is coding for accounts for this wrinkle very nicely. The fact is, it takes a reflectance profile containing two substantial energy peaks straddling that .40–.70 μm dead point at some distance on either side (and little or no energy elsewhere in the spectral window) to make our visual system respond with a magnitude approaching its responses to CA-ellipses generally. This explains why maximally saturated purples are always so dark, relative to the saturated versions of all the other colors. A maximally saturated purple requires a maximally tilted CA-ellipse whose high point is located at the dead point boundary here under discussion. But that high point is doomed to be misrepresented, by the visual system, as being lower than it really is, for the more we concentrate the incident reflectance profile's two energy peaks toward the dead point, the feebler the visual system's response. On the coding story here proposed, therefore, a maximally saturated purple is thus doomed to seem somewhat darker than any of the other saturated colors, at least to humans. And so it is.
All told, the structure of phenomenological space corresponds quite nicely to the structure of an antecedent space of specifiable objective features after all, namely, the space of possible CA-ellipses. As long as we portrayed reflectance profiles as so many lines meandering across a flat and everywhere-bounded two-dimensional space, the manner in which they cluster into objective similarity classes was almost certain to remain opaque. But once we roll that space into a horizontally unbounded tube, such matters become much easier to see. My central proposal, therefore, is that the objective physical feature that unites all of the reflectance-profile metamersFootnote 6 for any seen ‘commonsense’ color is the peculiar CA-ellipse that they all share as their best approximation. And our phenomenological color space maps the range of possible CA-ellipses very faithfully indeed, dimension for dimension, and internal location for internal location.
To see this directly, simply compare the space of possible CA-ellipses portrayed in Figure 6b with the long-familiar space of possible color sensations portrayed in Figure 2 (and also with the space of neuronal coding triplets portrayed in Figure 3c). Evidently, the differences are minor. First, the equator of the CA-ellipse space is not tilted up toward yellow, as is the equator of color-sensation space. This reflects, once again, the fact that the sensitivity curves of our three kinds of cone receptors are nonuniformly distributed across the human spectral window: the L- and M-cone curves overlap substantially. A saturated-yellow sensation (which requires a near-maximal external stimulation of both L- and M-cones) will therefore seem brighter than any other saturated-color sensation. And second, the CA-ellipse space is plainly ‘bulgy’ or more egg-shaped than the phenomenological spindle, as drawn in Figure 2. Figure 2 reflects the textbook orthodoxy of representing phenomenological color space as a double-coned spindle. But that portrayal is only a graphical convenience. Phenomenological color space, too, is more ‘bulgy’ than is conventionally portrayed in Figure 2, as has been known since Munsell first sought to portray it over a century ago. A more accurate portrayal would have it bulging outward somewhat, toward its top and bottom, which would bring its global structure even closer to the space of CA-ellipses portrayed in Figure 5a. Finally, a mathematical reconstruction of the shape of the human color solid, based on the Hurvich-Jameson model network mentioned earlier (see again Figure 3c), also yields a space that is like the double-coned spindle of Figure 2, but is rather bulgier toward the top and bottom extremes.Footnote 7
In all, our internal phenomenological color space is evidently a systematic homolog of the space of objective CA-ellipses. It is a reliable map of the global structure of that external feature space. Moreover, our ephemeral sensory indexings within that background map (i.e., our fleeting color sensations themselves) are moderately accurate indications of which CA-ellipse we might be confronting at any given moment. Finally, and most importantly, those CA-ellipses evidently constitute the resolution limit with which the human visual system can access the objective and often jagged reflectance profiles of objects. That resolution limit is fairly coarse, to be sure, but there is something objective that is being reliably, if rather fuzzily, resolved: reflectance profiles across the entire spectral window. We call them colors.
I should mention that the story just outlined is not the first attempt to find systematic similarities between the structure of our phenomenological color space and the structure of objective or physical color space. In a recent paper, L. D. Griffin (Reference Griffin2001) finds some notable similarities between the several ‘symmetry axes’ of the color spindle of Figure 2 and the ‘symmetry axes’ displayed in the less familiar CIE space (Commission Internationale de l'Éclairage) for objective colors widely used in the lighting industry. I believe that the parallels he finds are entirely genuine, if less comprehensive than the systematic structural isomorphism discovered on the present analysis. My only criticism is that he has chosen, as his representational target, the wrong space for objective color. The CIE space is a space for representing and analyzing illuminants, not reflectance profiles. It is a space for predicting the seen color that will result from mixing light at three utterly specific and canonical wavelengths, those corresponding to the focal λ sensitivities of the human S-, M-, and L-cones. It is a perfectly good and useful space, but it does not address the reality of the objective colors of the vast majority of objects in our terrestrial environment, which are almost exclusively reflectance colors, not self-luminous colors. Moreover, it fails to represent the all-important dimension of objective lightness and darkness captured by the space of possible CA-ellipses, as portrayed in Figure 6b. The CIE space has no room for black, for example, or for any of the darkish colors in the neighborhood of black. (The range of colors it comprehends corresponds most closely to a single horizontal cut through the equator of CA-ellipse space, a plane of constant brightness.) Nonetheless, Griffin's psychological/physical parallels are entirely welcome, for the colors of self-luminous bodies are as objectively real as the more common reflectance colors. (More on self-luminous colors below, in Section 8.)
5. Some Specific Tests
That the space of color sensation tracks (fairly closely) the space of CA-ellipses is quite evident. But it is still a hypothesis—if a plausible one—that what unites the (uniform-illumination) metamers for any given humanly perceivable color is the CA-ellipse that they severally share. (It is initially plausible because the coarse-grained resources of the human visual system typically cannot tell the difference between a given profile and its canonical approximation.) But let us quickly test the hypothesis against two salient examples of real metameric pairs, one drawn from Hardin (1988, 47) and one drawn from Fraser et al. (Reference Fraser2003, 30). The first example appears in Figure 7.
Figure 7.

These two reflectance profiles are metameric pairs, according to Hardin, despite their evident differences. How do they compare with regard to their respective CA-ellipses? To answer this question, I traced each of these profiles onto a separate transparency and rolled each into a cylinder. I then probed each profile (separately) with another rotatable cylinder slid inside it, a cylinder graduated with ellipses of varying tilt angles, until a ‘closest match’ was achieved, according to the criteria set out at the end of Section 3. (The relevant areas were measured by integrating over a substantial number of narrow, vertically oriented rectangles.) This yielded a unique CA-ellipse for each profile. The CA-ellipse for the double-peaked profile has a peak at a rotational position
 $R=.52$
μm, a height
 $H=14\% $
, and a tilt angle
 $T=17\% $
of maximum. The CA-ellipse for the single-peaked profile has a peak at a rotational angle
 $R=.535$
μm, a height
 $H=13\% $
, and a tilt angle
 $T=16\% $
of maximum.
The difference between these two CA-ellipses is
 $\Delta R=5\% $
,
 $\Delta H=1\% $
, and
 $\Delta T=1\% $
. This difference is marginal, and both CA profiles (with peaks very close to .53 μm) will present as a dull and quite dark green—barely distinguishable, if they are distinguishable at all.
The next pair of metameric profiles also present to us as green, though a somewhat brighter and more saturated green than in the preceding example. The taller of these two profiles (Figure 8) was probed in the manner described above and proves to have a CA-ellipse of
 $R=.53$
μm,
 $H=33\% $
, and
 $T=33\% $
of maximum. The second profile has a CA-ellipse of
 $R=.53$
μm,
 $H=29\% $
, and
 $T=35\% $
of maximum.
Figure 8.

The difference between them is
 $\Delta R=0\% $
,
 $\Delta H=4\% $
, and
 $\Delta T=2\% $
. Once again, the differences are marginal—at or close to the limits of human discrimination.
Given the systematic match already noted between our phenomenological color space (Figure 2) and CA-ellipse space (Figure 6b), these singular matches should come as no surprise. But it is salutary to check out the hypothesis (that the class of same-seeming metamers for humans corresponds very closely to the class of reflectance profiles that share the same CA-ellipse) against independent data.
6. An Important Objection
There remains a possible objection to my claim that our phenomenological color space is a (fairly high-resolution) map of CA-ellipse space and thus is a (rather low-resolution) map of the range of objective reflectance profiles. Hardin complains that our phenomenological color space displays an inescapable contrast between ‘unmixed’ colors (such as red or blue) and ‘mixed’ colors (such as orange or purple), a contrast that is completely absent in both the CA-ellipse space and in the objective space of possible reflectance profiles. How then can we identify colors with the latter?
Let us agree, at least for the sake of argument, that both parts of Hardin's claim are correct. This situation does nothing to undermine the claim that our phenomenological color space accurately maps the space of possible CA-ellipses, for the structure of the latter is plainly reflected, dimension for dimension, in the structure of the former. Hardin's antirealist argument here has got the ‘onus of match’ exactly backward. It is not incumbent on the domain portrayed to have every feature displayed by its portraying map: maps can display all sorts of features that are incidental to their role as effective maps (a common street map crumples easily and weighs about an ounce, e.g., in dramatic contrast to the urban domain that it portrays). The contrast between mixed and unmixed phenomenal colors is just such an incidental feature—an artifact, presumably, of the opponent process architecture of our color system.Footnote 8
What is required is that the relevant structure of the objective reality (namely, the three dimensions of variation for a CA-ellipse, as portrayed in Figure 6b) finds itself reflected in some structural features of the map that purports to portray that objective reality (namely, our phenomenological color spindle, as portrayed in Figure 2). In the present case, that requirement is plainly met. That the map might have other features that happen not to correspond to external structures is irrelevant.
My critique of Hardin's eliminativist position can perhaps be clarified with the following parallel, drawn from another modality. The human nervous system responds to temperature with two anatomically distinct types of receptor neurons: one for registering temperatures above the skin's temperature and another for registering temperatures below it. The first system produces a range of increasingly intense sensations all of which are similar to one another, and so does the second. But the family of sensations for warmth, on the one hand, and the family for coldness, on the other, are qualitatively quite distinct from each other. (No surprise, given that they arise from anatomically and physiologically distinct systems.)
Now, are we going to deny that objective temperature is identical with mean molecular kinetic energy on grounds that the objective scale of molecular kinetic energies embodies no such objective qualitative distinction between the regions above and below human skin temperature? Of course not. Nor should we hesitate, for similar (bad) reasons, to identify objective colors with reflectance profiles, on grounds that there is nothing in the domain of reflectance profiles that answers to phenomenological distinction between ‘pure’ and ‘mixed’ colors.
7. What, after All, Are Colors?
Even so, it remains to discuss exactly how our familiar objective colors should be fit into this emerging framework. Simply identifying the familiar range of colors with the evident range of CA-ellipses is a very poor option, since only a negligible proportion of material objects have a reflectance profile that is actually identical with the platonic perfection of a CA-ellipse. Any CA-ellipse, of course, projects back onto the original reflectance-profile space as a perfectly smooth, one-cycle sine wave of some altitude, amplitude, and left/right location within that space (see again Figure 5). But most objects will have a much noisier reflectance profile than a perfect one-cycle sine wave: the meandering metamers still dominate the reflectance profiles we actually encounter in the real world. Accordingly, identifying the various colors with the various reflectance profiles displayed by perfect CA-ellipses would have the consequence that almost nothing in the world is colored.
A much better option is to identify the full range of objective colors with the full range of objective reflectance profiles—both the relatively rare perfect CA-ellipses and the multitude of metameric profiles that severally cluster around them—and then acknowledge that we humans are able, with our native visual equipment, to perceive and discriminate those highly various reflectance profiles only at a rather low level of resolution. As we noted above, the CA-ellipse constitutes the limit of resolution at which humans can discriminate sameness and differences between objective reflectance profiles. In particular, we are typically unable to discriminate between any of the many metameric reflectance profiles that share the same ellipse as their canonical approximation. These mutually clustered metameric profiles will typically present themselves, to the casual human eye, as the same color, despite the residual but real differences between them.
This situation, however, is entirely unremarkable. The human auditory system, to take a related example, is skilled at recognizing and discriminating power-spectrum profiles within the acoustic spectrum. We are good at recognizing and discriminating the distinct voices of people familiar to us, the distinct voices of the various types of musical instruments, birds, animals, and so forth. No one will deny that distinct types of sounds are identical with distinct power-spectrum profiles displayed in a propagating wave train, and no one will deny that our auditory skills reside in the cochlea's ability to respond to those various profiles in an appropriately discriminatory fashion.
And yet, our cochlea has a resolution limit as well. Clustered around the distinctive power-spectrum profile of a typical oboe's middle A lies a multitude of possible “acoustic metamers,” all of them different from one another in ways that lie beneath the capacity of my cochlea to resolve. Despite their differences, they will all sound the same to me. And so also for any other familiar sort of sound. At a certain point, and inevitably, our discriminatory powers simply run out. Such acoustic metamers for familiar sounds are as real, and as inevitable, as the electromagnetic metamers for familiar colors.
But these undoubted facts about acoustic reality provide no grounds for irrealism or eliminativism about our commonsense ontology of sounds. Nor do the parallel facts, concerning electromagnetic metamers, provide grounds for irrealism or eliminativism about colors. Indeed, the ontological advantage, if any, should lie with colors. Sounds are ephemeral: a bird, a musical instrument, or an animal emits a sound only occasionally, and the sound fades (as
 $1/ r^{2}$
) to nothing as it promptly flees its point of origin. By contrast, a material body's electromagnetic reflectance profile is a quasi-permanent and stable property of that material body. It will change only if the molecular structure of the body's surface is modified in some way.
The stable solution then, to which we are thus attracted, is that the objective color of an object is identical with the electromagnetic reflectance profile of that object, within the window .40–.70 μm. Our native ability to recognize and discriminate such profiles is limited to recognizing and discriminating the altitude, tilt, and rotation angle of the CA-ellipse that approximates any given reflectance profile. But this native ability still gives us a highly reliable grip on an often-telling dimension of objective reality.
To be more specific, an object is a maximally saturated red, on this view, just in case its reflectance profile (however jagged and idiosyncratic) has a CA-ellipse of altitude 50%, a maximum tilt, and a rotation position with the ellipse's highest elevation at .63 μm (see Figure 9a). An object is a somewhat dull yellow, on this view, just in case its reflectance profile has a CA-ellipse of altitude 50%, a moderate tilt, and a rotation position with the ellipse's highest elevation at .58 μm (see Figure 9b). And so forth for every other objective color, no matter what its lightness, degree of saturation, and peculiar hue (see Figures 9c–f). We might think of this as the “wobbling penny” account of the space of possible reflectance profiles, for that is how the CA-ellipse variously appears for diverse reflectance profiles.
Figure 9.

This position has the consequence that two distinct objects, both of which are a maximally saturated yellow (or any other color), need not be exactly the same color, for they may sport distinct metamers included within the class of maximally saturated yellows. They are both genuine instances of maximally saturated yellow, let us assume, but they may be different instances of what (as we now appreciate) is an interestingly diverse class. This description is, to be sure, a significant departure from our normal modes of speech, because common sense innocently assumes that there are no color differences underneath what our eyes can discriminate in broad daylight. But this naïve assumption must be let go. And the existence of diverse reflectance-profile metamers is precisely what demands its surrender. Even so, the existence of colors themselves, as objective features of objects, is not threatened. We simply have to acknowledge that there is slightly more to color than “meets the human eye,” even under the optimal conditions of broad daylight.
It is interesting that hidden diversity and sameness of objective colors are not entirely inaccessible to the human visual system. A simple trick will make such matters visually available, even to one who is color-blind. Given two shirt buttons, of apparently the same yellow color to normal vision, one can determine whether (1) they are exactly the same color (i.e., have identical reflectance profiles) or (2) merely have distinct metameric variants on a general yellow theme. We can do this by running both buttons, side by side, through the gauntlet of a rainbow projected on a wall. If we project a beam of sunlight through a prism in an otherwise darkened room, we will produce a fan of distinct monochromatic wavelengths to serve as diagnostic probes of each button's reflectance at any given wavelength of light. If the two buttons do share identical reflectance profiles, then their joint appearance to the human eye will vary, of course, as they are marched through the fan of distinct diagnostic illuminants. But at each position against the fan they will always display the same appearance as each other. By contrast, if the buttons have distinct metameric variants on yellow, then at one or more points in their joint journey across the rainbow they will appear different from one another.They must. That they have distinct reflectance profiles entails that they will display differential reflectance behavior at some one or more points within the visible spectrum. Even a color-blind person will detect such discrepancies in their objective reflectance behaviors, since they will still present themselves, to him, as visible differences in apparent grayscale brightness. In this way the “hidden” color metamers are made visible, even to people who are color-blind.
Collateral or background information can also be a reliable guide to judging whether two same-seeming objects really have identical reflectance profiles or merely share the same ellipse as their canonical approximation. If one is viewing two visually identical dark-red cherries or two visually identical yellow bananas, for example, one can be confident that the two cherries have genuinely identical reflectance profiles, and so also for the two bananas. For one can be independently confident that the two ripe cherries have identical molecular constitutions at their surfaces, and so also for the two ripe bananas. Such identity in molecular constitution physically guarantees identity in their reflectance profiles. However, when background information suggests a quite different molecular constitution for two same-seeming objects—as with a purple plum and a patch of purple paint—the distinct-metamers hypothesis will have a better claim on the situation.
8. The Diversity of Objective Colors
It remains to highlight the contrast between the familiar reflectance colors, as characterized in the preceding pages, and the less common emittance or self-luminous colors, as displayed in a fire, a star, an incandescent bulb, or an LED (light-emitting diode). The former is a matter of what profile of light an object reflects; the latter is a matter of what profile of light an object emits. Whatever common sense might think, these are entirely distinct properties. One and the same object can simultaneously possess incompatible ‘colors’ of each kind, as when a stove top heating element veridically presents its familiar reflectance color—a dark charcoal gray—when the kitchen lights are on; but when the lights are switched off and the room is plunged into darkness, the element reveals its self-luminous or emittance color of dull red (the relevant dial on the stove's control panel was set at “low” all along). Though we could not see its self-luminous color in the first condition—because the intensity of the reflected light swamped the comparatively faint emitted light—the darkened condition allows that self-luminous color to become visible.
Self-luminous colors were an extremely rare occurrence in the evolutionary environment that gave birth to our current color vision. Only the sun, the stars, the occasional firefly, and the occasional forest fire ever displayed a self-luminous color. Accordingly, and apart from the character of solar radiation as a background illuminant, the self-luminous colors must have played a negligible role in the evolutionary selection of the enabling mechanisms for human color vision. In modern society, of course, the self-luminous colors have become commonplace. And in fact, where metamers are concerned, the self-luminous colors are somewhat better behaved than the reflective colors. The colors of a thermally incandescent object almost always present a smoothly varying emittance profile, whose peak magnitude is tightly tied to the object's absolute temperature. And the self-luminous color of an object engaged in spectral emission (i.e., in photon emission from electron-shell transitions) is almost always a matter of one or more narrow spikes of monochromatic light (as from an LED or a sodium street lamp), which color is a reliable guide to the object's peculiar atomic constitution. Metamers are entirely possible here, as elsewhere, but in fact they are much less common for self-luminous colors than for reflectance colors.
The objective space for self-luminous colors (in the window .40–.70 μm) is slightly but importantly different from the objective space for reflectance colors. In particular, the vertical dimension of the relevant cylinder represents, not reflective efficiency (which tops out at 100%), but emission intensity, which has no upper limit. Nonetheless, our native representational space (specifically, the color-coding neuronal activation space of Figure 3c) does its best to represent this relatively new range of possible emittance profiles, using its existing resources of brightness, saturation, and hue. But here it encounters an anomalous situation, in that the brightness levels of typical self-luminous objects are much too high to be accounted for in terms of a 100% reflectance efficiency across the spectrum (i.e., as originating from a maximally reflective white object), and they often display a vivid hue (i.e., a nonwhite color) in any case. The human visual system responds by coding such anomalous (i.e., self-luminous) inputs at an appropriate place on the ceiling of our opponent-cell activation space, but outside the point-like apex of the spindle-shaped volume that confines all the representation points for the less dramatic reflectance colors (see Figure 3c).
These ceiling positions are “impossible” positions, as far as the reflectance colors are concerned. (No reflectance color can be as bright as the brightest possible white and yet be something other than white.) But by that very fact, those unusual ceiling positions serve as reliable diagnostic positions, in our preexisting neuronal activation space, to indicate the presence of a self-luminous object and to indicate its peculiar hue and saturation. An information-processing system that was shaped by evolution to recognize and discriminate one kind of color turns out to be able to recognize and discriminate a second kind of color as well, and to do so in a manner that can sharply distinguish both.
Precisely because they are typically coded, by the visual system, outside the normal phenomenological color spindle, the self-luminous colors typically stand out like beacons against the darkness.Footnote 9 Their typical representational space is the two-dimensional ceiling of the opponent-cell activation space. Save for a single point at its center, this space is entirely distinct from the three-dimensional volume of the familiar spindle-shaped solid for representing the reflectance colors. But it, too, maps moderately well onto the objective range of its proprietary properties, namely, the various emittance profiles displayed by self-luminous bodies. (Exactly how the visual system discriminates between the different brightness levels of the self-luminous colors—note that the ceiling of the opponent-cell space has only two dimensions—is a matter still unclear on the present account. But I shall leave its pursuit for another occasion.)
I conclude that there are at least two quite distinct kinds of objectively real colors, the reflectance colors and the self-luminous colors. The objective structure of each domain of properties becomes evident if one rolls the window of the visible spectrum into an abstract cylinder and then examines the space of possible planar cuts through that cylinder, as providing the best approximation of the fine-grained details of the possibly noisy power spectrum profile currently portrayed around its surface. For reflectance colors, the space of possible planar cuts (i.e., the space of possible CA-ellipses) is homomorphic with the spindle-shaped solid of our phenomenological space. And for the more ostentatious self-luminous colors, the space of their possible hues and saturations is homomorphic with the space of possible activations within the otherwise unused two-dimensional ceiling of the opponent-cell activation space (see again Figure 3c). The colors, of both kinds, are thus entirely real and are as objective as you please. We can see them both, for in most cases we can recognize and discriminate both reflectance profiles and emittance profiles, and discriminate the one from the other. The only disappointment here is both negligible and inevitable: some of the fine-grained structure of both kinds of profiles lies beneath the resolution of our native visual system. But this is no argument for irrealism about those profiles (of course), nor is it an argument for irrealism about colors. For that is precisely what the two kinds of colors are: reflectance profiles and emittance profiles, respectively.
9. Comparison with a Related View
The account of objective colors defended above shares many of the same motivations and some of the positive substance of the realist account of colors recently urged by Byrne and Hilbert (Reference Byrne and Hilbert2003). But some important differences stand out, and I will close by bringing several of them to your attention. First, and perhaps least, those authors propose a new notion of a ‘determinate color’ (e.g., ‘determinate red’) whose extension is exactly the set of metameric reflectance profiles between which the human visual system is unable to distinguish. By contrast, I propose to identify distinct colors with distinct reflectance profiles and then embrace the consequence that the human visual system cannot distinguish all color differences, since it cannot distinguish all reflectance profile differences. We see color similarities and differences only down to the resolution limit defined by the range of possible CA-ellipses. There are color similarities and differences beneath what we can detect just by looking. Our existing color vocabulary, therefore, comprehends only a coarse partitioning of the objective reality. Nevertheless, that partitioning is still objective in character and is highly useful as a guide to many of the causal properties of material objects.
Second, and much more important, Byrne and Hilbert acquiesce in the received wisdom that the family of metamers for any commonsense color displays no unifying intrinsic feature specifiable in purely physical terms. They should not have acquiesced to this claim, because we can indeed specify, in terms “of interest to a physicist,” the feature that unites the family of metamers for a given commonsense color: they all share the identical reflectance-space ellipse as their canonical approximation. Moreover, this shared objective feature is precisely what gets mapped within the human subjective or phenomenological color space. Accordingly, we can see how the space of human color sensations counts as a structurally accurate map of an objective domain of properties, a real achievement by our visual system that remains either denied or unrecognized in their view.
Finally, Byrne and Hilbert attempt to salvage a unitary conception of color by attempting to knit together the distinct features of reflectance, emittance, and transmittance into a single and deliberately more general notion of productance. By contrast, the view of this essay tends in exactly the opposite direction. I claimed earlier that reflective colors are a family of properties genuinely distinct from the family of self-luminous colors. And I will say the same for a third family of ‘color’ properties: the various profiles of transmittance displayed by transparent and translucent objects such as colored glass, colored liquids, and some gemstones. All three types of color are features to which the human visual system gives us some nontrivial perceptual access, and in each case, that perceptual access involves our capacity to distinguish the power-spectrum profiles of the electromagnetic radiation arriving to our eyes. But the three types of objective properties themselves (reflectance, emittance, and transmittance) are radically distinct, from the point of view of informed physics. It would be folly to try to conflate them all into a single notion, especially when we already enjoy a perceptual system that allows us to spontaneously recognize the distinctions between them on a fairly reliable basis.
To add further force to this argument, the varieties of objective ‘chromatic phenomena’ do not end with the three types just mentioned. We must reckon also with the range of ‘scatterance colors’, as instanced in the ‘blue’ of the daytime sky. There are also ‘interference colors’, as displayed, for example, in various thin films such as an oil slick floating on water. There are also ‘refractance colors’, as get displayed when sunlight hits a prism, a many-faceted gemstone, or a spray of spherical water droplets. These three additional kinds of color also involve importantly different intrinsic properties, features, or mechanisms for interacting with light, each in their own characteristic way.
If we want to respect the impulse toward objectivity implicit in the commonsense conviction that the colors are real features of the external world, we should respect the lessons of modern physics that ‘color properties’ come in a substantial variety of objectively distinct families. We are merely stuck with a single perceptual modality—a trichromatic visual system—with which to ply access to all of them. But that is no grounds for conflating the distinct types of objective color themselves. They are importantly different from one another, even in the details of their visual appearance. Withal, and however various, those distinct types of color remain as real and as objective as you please, despite what commentators from Locke to Hardin have too hastily insisted. The colors—all six distinct families—deserve to be welcomed back into the fold of objectively real properties. We just need to understand them a little differently.