Introduction
The end-Permian mass extinction was the most taxonomically and ecologically severe extinction in the history of animal life, eliminating 79% of all marine animal genera (McGhee et al. Reference McGhee, Sheehan, Bottjer and Droser2004; Payne and Clapham Reference Payne and Clapham2012). Following the extinction, many marine taxa appear to be smaller than those before the event (Schubert and Bottjer Reference Schubert and Bottjer1995; Twitchett Reference Twitchett1999; Fraiser and Bottjer Reference Fraiser and Bottjer2004; Pruss and Bottjer Reference Pruss and Bottjer2004; Payne Reference Payne2005; Luo et al. Reference Luo, Lai, Jiang and Zhang2006; He et al. Reference He, Shi, Feng, Campi, Gu, Bu, Peng and Meng2007; Twitchett Reference Twitchett2007; Luo et al. Reference Luo, Lai, Shi, Jiang, Yin, Xie, Tong, Zhang, He and Wignall2008; He et al. Reference He, Twitchett, Zhang, Shi, Feng, Yu, Wu and Peng2010; Metcalfe et al. Reference Metcalfe, Twitchett and Price-Lloyd2011; Payne et al. Reference Payne, Summers, Rego, Altiner, Wei, Yu and Lehrmann2011; Song et al. Reference Song, Tong and Chen2011). Because an organism’s size plays a key role in its physiology, life history, and ecology (Peters Reference Peters1983; Calder Reference Calder1984; Schmidt-Nielsen Reference Schmidt-Nielsen1984; Brown Reference Brown1995), the small size of Early Triassic marine animals may hold important clues regarding the extinction and recovery processes beyond what can be learned from the study of taxonomic diversity. However, the recent discovery of gastropod specimens from the Smithian and Spathian substages of the Early Triassic larger than any previously known suggests that the magnitude and duration of Early Triassic size decrease may have been vastly overestimated (Brayard et al. Reference Brayard, Nützel, Stephen, Bylund, Jenks and Bucher2010; Brayard et al. Reference Brayard, Nützel, Kaim, Escarguel, Hautmann, Stephen, Bylund, Jenks and Bucher2011). But because long-term patterns of size evolution in most well-fossilized taxa have never been documented, the actual magnitude and duration of size change during and after the end-Permian mass extinction remains poorly known and the underlying mechanisms incompletely understood.
The phenomenon of size decrease associated with extinction events has been called the “Lilliput Effect,” after the island of miniature people in Jonathan Swift’s Gulliver’s Travels (Urbanek Reference Urbanek1993; Harries and Knorr Reference Harries and Knorr2009). Such size decreases have occurred in various animal groups after mass extinction events, and a pattern of size reduction may be common to major biotic crises (Arnold et al. Reference Arnold, Kelly and Parker1995; Smith and Jeffery Reference Smith and Jeffery1998; Twitchett and Barras Reference Twitchett and Barras2004; Lockwood Reference Lockwood2005; Twitchett Reference Twitchett2007; Harries and Knorr Reference Harries and Knorr2009; Huang et al. Reference Huang, Harper, Zhan and Rong2010). Urbanek (Reference Urbanek1993) originally used the term “Lilliput Effect” to describe the temporary size reduction of a surviving species in the aftermath of an extinction event. Here, we are concerned with post-extinction size change more broadly, which may result from (1) within-lineage evolution toward smaller sizes, (2) extinction of larger species, or (3) origination of smaller species. These three modes of size change can operate individually or in concert to shift the overall size distribution of a biota. Because large body size tends to be correlated with small population size, larger species are often assumed to be at greater risk of extinction (e.g., Stanley Reference Stanley1986; Brown Reference Brown1995). Therefore, we might expect that size-selective extinction among lineages would be a likely mechanism of size reduction at extinction events. On the other hand, some taxa exhibit a component of within-species or within-genus evolution toward smaller size across extinction horizons (Smith and Jeffery Reference Smith and Jeffery1998; Twitchett Reference Twitchett2007; Morten and Twitchett Reference Morten and Twitchett2009). The relative importance of within-lineage processes and among-lineage processes (size-biased extinction and origination) has received little attention (Rego et al. Reference Rego, Wang, Altiner and Payne2012).
There is substantial evidence for size decrease between the Late Permian and Early Triassic, but there has been little quantitative comparison of size change globally across major clades. Schubert and Bottjer (Reference Schubert and Bottjer1995) first noted the small sizes of Early Triassic gastropods in the western USA. Fraiser and Bottjer (Reference Fraiser and Bottjer2004) compiled the first quantitative record of Early Triassic gastropod sizes, finding no gastropods larger than 2 cm in the Sinbad Limestone of southeastern Utah, in contrast to comparable assemblages from the Middle Permian of southwestern USA and the Middle Triassic of south China. Compiling a global database of gastropod size based on literature review, Payne (Reference Payne2005) showed the loss of large gastropods in the earliest Triassic, with small sizes persisting until the Middle Triassic. This pattern of size reduction has also been documented in trace fossils. In the Werfen Formation of northern Italy, Twitchett (Reference Twitchett1999, Reference Twitchett2007) recorded a decrease in both maximum and mean burrow diameter by approximately an order of magnitude across the Permian/Triassic boundary. Pruss and Bottjer (Reference Pruss and Bottjer2004) measured the diameter of trace fossils in the Early Triassic Virgin Limestone of southern Nevada and eastern California; though there was not enough data to assess the magnitude of size change, their results suggest Early Triassic trace fossils are smaller than their Permian and Middle Triassic counterparts. In addition to gastropods and trace fossils, Early Triassic size reduction has been reported in the sizes of the brachiopod Lingula from the Werfen Formation of northern Italy (Metcalfe et al. Reference Metcalfe, Twitchett and Price-Lloyd2011), foraminiferans from Meishan, Liangfengya, and Shangsi sections in south China (Song et al. Reference Song, Tong and Chen2011), as well as mean (but not maximum) bivalve size in collections from the Natural History Museum, London (Twitchett Reference Twitchett2007). Size reduction also occurred during the mass extinction event in the latest Permian (Changhsingian) of south China; bed-by-bed measurements of brachiopods from Meishan, Dongpan, and Majiashan sections (He et al. Reference He, Shi, Feng, Campi, Gu, Bu, Peng and Meng2007; He et al. Reference He, Twitchett, Zhang, Shi, Feng, Yu, Wu and Peng2010) and conodonts from Meishan and Shangsi sections (Luo et al. Reference Luo, Lai, Jiang and Zhang2006; Luo et al. Reference Luo, Lai, Shi, Jiang, Yin, Xie, Tong, Zhang, He and Wignall2008) show many instances of size decrease, but instances of size increase as well.
One limitation to our understanding of Early Triassic size evolution is that most of the evidence comes from analyses based on data from individual stratigraphic sections. At the local scale, it may be difficult to distinguish facies effects from global patterns of size change. A compilation of size data from specimens around the world would enhance our understanding of global trends in body size. A further limitation to our understanding of Early Triassic size evolution is that only a few invertebrate clades have been studied quantitatively. Just as extinction selectivity can shed light on the causes of extinction (Knoll et al. Reference Knoll, Bambach, Payne, Pruss and Fischer2007), differential patterns of size evolution among clades can illuminate processes controlling size reduction and recovery.
As a complement to this previous work, in this study we use data from the literature to build a global picture of size change in multiple clades. We compare patterns of size change from Late Permian through the Early Triassic across eight diverse marine clades: gastropods, bivalves, calcitic and phosphatic brachiopods, ammonoids, ostracods, conodonts, and foraminiferans. These taxa differ in terms of life habit, motility, size, diversity dynamics, feeding methods, trophic level, skeletal mineralogy, skeletal buffering, and efficiency of circulatory and respiratory systems. Consequently, similarities and differences in size evolution may shed light on the key environmental or biotic controls on extinction and recovery beyond what has been learned from analyses of taxonomic diversity and environmental context alone.
Data and Methods
Data Collection
We constructed a database containing size measurements for global fossil occurrences of eight marine clades spanning the Late Permian (Wuchiapingian) through Middle Triassic (Ladinian). The database includes 11,224 specimens representing 445 gastropod species, 194 bivalve species, 534 calcitic brachiopod species, 16 phosphatic brachiopod species, 907 ammonoid species, 116 ostracod species, 270 conodont species, and 261 foraminiferan species. We gathered size data from the published taxonomic literature, mostly monographs and single-locality to regional studies. We collected fossil specimen measurements directly from tables or text, or measured specimens from scaled figures using digital calipers. Monograph-derived size data have been shown to be a reasonable proxy for bulk sample populations (although typically recording the larger specimens from a collection) and a valuable data source for macroevolutionary size trends (Kosnik et al. Reference Kosnik, Jablonski, Lockwood and Novack-Gottshall2006; Krause et al. Reference Krause, Stempien, Kowalewski and Miller2007). Taxonomic identifications were standardized following recent publications for each clade.
The eight marine taxa in our database are ideal for comparing size-evolution trends among clades through the end-Permian mass extinction and subsequent Triassic recovery. We chose well-fossilized marine groups with a good record from the Late Permian through Middle Triassic. In addition, we chose clades with fossil size measurements that can be directly related to the size of the whole organism. We focused on higher taxa that produce one or two skeletal elements that are a good proxy for that taxon’s soft tissue mass. Though conodonts have many skeletal elements, here we use P1 elements as a proxy for the size of the conodont animal. For a variety of animal groups, tooth size correlates with body weight over many orders of magnitude and is commonly used to predict body size in fossils (Randall Reference Randall1973; Gingerich et al. Reference Gingerich, Smith and Rosenberg1982). Tooth size and body length are correlated in hagfish and lampreys, the closest extant relatives of the conodonts (Krejsa et al. Reference Krejsa, Bringas and Slavkin1990). Though this relationship cannot be established quantitatively for conodont animals due to the lack of complete body fossils, it is likely to hold; larger conodont animals certainly had larger elements (Purnell Reference Purnell1994; Gabbott et al. Reference Gabbott, Aldridge and Theron1995).
Data Analysis
For our analyses, we used the maximum linear dimension (in log10 mm) recorded for each species in a given time interval. Log transformation of data is standard for studies of body size distributions and evolutionary rates (e.g., Gingerich Reference Gingerich2009). We chose maximum linear dimension as a size measure because it is a simple, accurate proxy for biovolume (Niklas Reference Niklas1994; Novack-Gottshall Reference Novack-Gottshall2008) that is typically available even in cases where all three major axes are not reported or illustrated, thus maximizing taxonomic coverage. Using only the maximum size per species avoids the influence of juvenile specimens in the database and is common practice for studies of body size (Stanley Reference Stanley1973; Jablonski Reference Jablonski1997; Lockwood Reference Lockwood2005). Maximum specimen size is a reasonable metric for species size because size variation within species is very small relative to that among species (Dommergues et al. Reference Dommergues, Montuire and Neige2002; Payne Reference Payne2005). After culling smaller species measurements, there are 3,189 unique species-stage combinations in the dataset.
We binned time as geologic stages (Wuchiapingian through Rhaetian) because it was the finest temporal resolution that allowed us to retain most of the data. All subsequent analyses are done on species-level data at the time resolution of stages. Species-level stratigraphic ranges are based on our observed data.
Median Size
Comparing size change across the eight marine clades, we focused on two metrics of body size distribution: (1) median and (2) maximum size per stage. Median size is highly correlated with mean size in our dataset and is less sensitive to outliers than the mean. We used Mann-Whitney U-tests to determine whether size data from two stages were consistent with samples drawn from the same underlying distribution, or if the distribution of sizes was significantly different between time intervals (different medians between groups). We used the Mann-Whitney test rather than a t-test to be conservative in the identification of significant changes in the central tendency, even though most of the log-transformed size distributions are close to normal.
Maximum Size
We compared maximum sizes between stages for each clade using both raw data and data subsampled to a uniform number of species. Subsampling was required to assess whether changes in the observed maximum size could be explained simply by reductions in observed diversity or whether they required additional explanation. In this analysis, we were agnostic as to whether changes in observed diversity resulted from loss of true diversity, which was almost certainly the case across the Permian/Triassic boundary, versus smaller sample size due to changes in rock availability, interval duration, researcher interest, or other factors. For each clade in each time interval we subsampled the size distribution (with replacement) to the number of species in the stage with the lowest observed diversity. We repeated this procedure 10,000 times for each clade in each stage to obtain an expected distribution of maximum sizes after correcting for observed diversity.
Components of Size Change
Change in the overall mean size across species could occur through size-biased extinction, within-species changes in size, and/or through size-biased origination. We investigated the extent to which these three components of size change contributed to the total change in mean clade size across the boundary following the methodology of Rego et al. (Reference Rego, Wang, Altiner and Payne2012). The total change in mean clade size is the difference between the mean size of all species in a given stage (T2) and the mean size of all species in the preceding stage (T1). For each clade, we divided the species in the earlier stage (T1) into the extinction victims of the earlier stage and those that survived into the subsequent stage (T2); the species in the later stage (T2) were likewise separated into survivors from the preceding stage and species originating in the later stage (T2). To determine the within-lineage evolution component of size change, it was important to have size measurements for the surviving species from both before and after the boundary. The change in mean size due to size-biased extinction, Δex, is equal to T1S–T1A, where T1S is the mean size of survivors in stage T1, and T1A is the mean size across all species (survivors and victims) in stage T1. The change in size due to within-lineage evolution, Δlin, is equal to T2N–T1S, where T2N is the mean size of the non-originators (i.e., the survivors from stage T1) as measured in stage T2. The change in mean size due to size-biased origination, Δor, is equal to T2A–T2N, where T2A is the mean size of all species (survivors plus originators) in stage T2. The overall change in mean clade size between T1 and T2 is thus partitioned into a size-biased extinction component Δex, a within-lineage evolution component Δlin, and a size-biased origination component Δor (i.e., mean[T2] – mean[T1]=Δex+Δlin+Δor). We emphasize that we are not calculating metrics of victim or originator size, nor comparing the mean size of victims or originators to other species in the interval. Instead, Δex, Δlin, and Δor are estimates of the effect that size-biased extinction and origination, and within-lineage evolution, have on the observed size change.
Results
Figure 1 illustrates the species-level size history of the eight marine clades studied here. Most clades decreased in both maximum and median size from the latest Permian (Changhsingian) to earliest Triassic (Induan) (Fig. 1). The major exception to this pattern is the ammonoids, which increased in median size from the latest Permian to the earliest Triassic. After the Induan (earliest Triassic), many clades increased in maximum or median size during Olenekian (late Early Triassic) and Anisian (early Middle Triassic) time.
Species-level size data for the eight marine clades from the Late Permian through the Late Triassic (x-axis stage abbreviations: Wu=Wuchiapingian, Ch=Changhsingian, In=Induan, Ol=Olenekian, An=Anisian, La=Ladinian, Ca=Carnian, No=Norian, Rh=Rhaetian). The gray bars highlight the Permian-Triassic transition (Changhsingian and Induan stages). Note that the eight plots have different scale ranges on the y-axes. Each boxplot displays the median, 25th percentile, and 75th percentile, with whiskers extending to the 5th and 95th percentiles.

Median
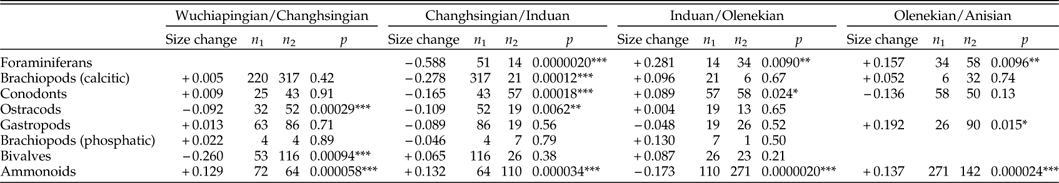
Six out of the eight marine clades decreased in median size from Late Permian to Early Triassic (Changhsingian to Induan stages; Fig. 2), with foraminiferans, calcitic brachiopods, conodonts, and ostracods exhibiting statistically significant declines (Table 1). The two exceptions are the bivalves, which show a non-significant (Mann-Whitney U-test, p=0.38, two-tailed test) increase in median size, and the ammonoids, which experienced a highly statistically significant (Mann-Whitney U-test, p=0.000034) increase in median size.
Trends in median size of each clade through time (stage abbreviations are the same as in Fig. 1). The gray bar highlights the Permian-Triassic transition (Changhsingian and Induan stages). In order to compare size trends between clades of vastly different sizes, we rescaled the data such that the average of the stage-level mean values for each clade was set to a value of zero. Thus, zero on this graph represents the long-term average value for each clade. We used this approach rather than calculating the average of all species measurements so that stages with more species did not have an unequal pull on the clade mean size, but either method yields the same relative size changes between clades.
Change in clade median size (in log10 mm) across stage boundaries, the number of specimens (species) in the stage before the boundary (n 1) and after the boundary (n 2), and the significance level of a Mann-Whitney U, two-tailed test (p) (* denotes p≤0.05; ** p≤0.01; *** p≤0.001).
Not only do most clades show a prominent size reduction from the Changhsingian to the Induan, but all clades except for the ammonoids and conodonts were also well below their long-term mean size in the Induan. In fact, four of the eight clades show their smallest median size of the entire study interval in the Induan (Fig. 2). No stage other than the Induan contains more than one overall clade minimum in median size. Given 51 clade-stage combinations with eight overall clade minimum sizes, the probability of observing four overall clade minima in the Induan is 0.021 (binomial test), indicating that the size minima within these clades are non-randomly clustered in this time interval. In contrast, the ammonoids reached large median size in the Induan: larger than the rest of their Permian-Triassic size history (Fig. 2).
Maximum
Figure 3 shows trends in maximum size both before (Fig. 3A) and after (Fig. 3B) standardizing for changes in observed species diversity. Seven out of eight clades decreased in maximum size from the latest Permian to earliest Triassic (Fig. 3A); this is a significant concentration of size decreases in the Induan compared to the overall frequency of size decreases in our dataset (binomial test, p=0.015). The one clade that did not decrease in maximum size across the Permian/Triassic boundary (PTB) is the clade for which we have the least amount of data (only 16 species): the phosphatic brachiopods, which show very little change in maximum size. In contrast, calcitic brachiopods, foraminiferans, gastropods, and bivalves experienced particularly large reductions in maximum size across the PTB. Ostracods decreased notably in maximum size both going into the Changhsingian (with the disappearance of the large Myodocopids) and across the extinction horizon. These five clades show their lowest maximum size of the whole study interval in the Induan. Although ammonoids and conodonts decreased slightly in maximum size across the PTB, the change was small compared to their size variation later in the Triassic. The Permian/Triassic boundary was not an interval of notable maximum size change for these two clades.
A, The maximum size for each clade through time (stage abbreviations are the same as in Fig. 1). The gray bars highlight the Permian-Triassic transition (Changhsingian and Induan stages). As in Fig. 2, sizes are normalized to each clade’s mean size in order to compare relative size change among clades. B, The median of resampled maximum size values for each clade through time; each stage was subsampled 10,000 times with replacement to match the smallest number of species per stage for that clade.
Figure 3B shows the medians of the maximum body size values after 10,000 replicate subsamples to a standardized value of taxonomic diversity. Overall, sample-standardization does not notably alter the trends in maximum size illustrated in Figure 3A, and the size decrease in the Early Triassic still stands out as a major shift in size distributions. Even after subsampling, the frequency of size decreases in the Induan is significantly higher than the expectation from all stages (binomial test, p=0.0090). In addition, significantly more clades show their smallest maximum size of the entire study interval in the Induan than expected for all stages (six out of eight clades, after subsampling; binomial test, p=0.00030).
Components of Size Change
Figure 4 presents the size distributions of Permian/Triassic boundary victims, survivors, and originators, as well as the contribution of the three components of size change to the Early Triassic size reduction (Fig. 4, rows labeled Ch/In). Only calcitic brachiopods, foraminiferans, conodonts, and bivalves had enough species survive into the earliest Triassic (that were measured both in the Changhsingian and the Induan) to evaluate the component of within-lineage size change. Either within-lineage size evolution did not play a large role in the other marine groups, or its signal is masked by surviving species changing taxonomic name across the boundary (i.e., pseudoextinction). The bivalves had little overall change in mean size across the boundary, and so the three components of size change balance each other out (Δex+Δlin+Δor is near zero). For the clades that show mean size decrease across the boundary, large species preferentially going extinct (size-biased extinction) appears to be an important factor for size reduction in brachiopods. However, foraminiferans and conodonts both show strong within-lineage size decrease in the extinction survivors. In fact, most of the Early Triassic size reduction in these two clades resulted from within-lineage evolution toward smaller sizes, rather than size-selective extinction or origination. Across the marine clades studied, it is clear that multiple modes of size change contributed to Early Triassic size reduction.
Relative magnitude of the three components of size change (size-biased extinction, within-lineage evolution, and size-biased origination) from the Late Permian through the Middle Triassic (stage abbreviations are the same as in Fig. 1). Bottom row: An example of the source data for the “Ch/In” row of bar graphs above; for each clade, each set of four dotplots show the size distribution of extinction victims in the Changhsingian (dark gray), survivors (boundary crossers) as measured in the Changhsingian (black), survivors as measured in the succeeding stage (black), and new originators in the succeeding stage (light gray). Horizontal gray lines denote the mean of each distribution. Top three rows: For each stage boundary and clade, bars denote magnitude of size change accounted for by size-biased extinction (dark gray), within-lineage evolution (black), and size-biased origination (light gray), calculated as described in text. The relative magnitude of the three components cannot be calculated when survivor species are not measured both before and after the stage boundary and so the bar graphs have been left out for cases where there were not size measurements for survivors for both relevant stages.
Timing and Mode of Size Recovery
Most marine clades show size reduction across the Permian/Triassic boundary, but how long does this effect last? Some marine groups, such as the calcitic brachiopods did not regain pre-extinction sizes within the study interval, but most show at least some size recovery (Fig. 1). To summarize the direction of size change through time, Table 1 charts the sign of size change in clade medians between stages. The transition from the latest Permian (Changhsingian) to earliest Triassic (Induan) shows more significant size reduction than any other interval. Table 1 also suggests that size recovery was already starting in the late Early Triassic (Olenekian), followed by significant size increases going into the Middle Triassic (Anisian). Where we have data for the Anisian, many marine groups have already returned to their pre-extinction size distributions. Thus, the predominance of unusually small body sizes was mostly restricted to Induan time.
Size increase during the Olenekian and Anisian resulted from a combination of the three components of size change (Δex, Δlin, and Δor). Figure 4 shows the extent to which size-biased extinction, within-lineage evolution, and size-biased origination contribute to the size recovery (Fig. 4, rows labeled In/Ol and Ol/An). What is striking is the inconsistent magnitudes of the three components between clades during size recovery. In some cases, size-biased origination plays a large role in overall mean size increase (e.g., Induan/Olenekian brachiopods and conodonts), in other cases within-lineage size increase is the dominant factor (e.g., Induan/Olenekian foraminiferans and bivalves) and in others, a combination of size factors are at work (e.g., Olenekian/Anisian foraminiferans). Like Early Triassic size decrease, size recovery is accomplished through multiple modes of size change.
Discussion
Size Dynamics during Extinction and Recovery
Early Triassic size reduction has been described for various marine organisms, but much previous work has focused on only a few invertebrate clades and localities (Schubert and Bottjer Reference Schubert and Bottjer1995; Twitchett Reference Twitchett1999; Fraiser and Bottjer Reference Fraiser and Bottjer2004; Pruss and Bottjer Reference Pruss and Bottjer2004; Payne Reference Payne2005; Luo et al. Reference Luo, Lai, Jiang and Zhang2006; He et al. Reference He, Shi, Feng, Campi, Gu, Bu, Peng and Meng2007; Twitchett Reference Twitchett2007; Luo et al. Reference Luo, Lai, Shi, Jiang, Yin, Xie, Tong, Zhang, He and Wignall2008; He et al. Reference He, Twitchett, Zhang, Shi, Feng, Yu, Wu and Peng2010; Metcalfe et al. Reference Metcalfe, Twitchett and Price-Lloyd2011; Song et al. Reference Song, Tong and Chen2011). We find the pattern of size decrease after the end-Permian extinction extends to multiple major marine groups on a global scale. New fossil measurements in the Olenekian have called into question the extent and duration of post-extinction size decrease (Brayard et al. Reference Brayard, Nützel, Stephen, Bylund, Jenks and Bucher2010). However, the fact that we find evidence for size decrease from the Changhsingian to the Induan in most taxa suggests that size reduction was a real phenomenon, if perhaps shorter-lived than previously assumed. The size decrease occurred in clades that differ greatly in body size, from decimeter-scale bivalves and gastropods to sub-millimeter-scale foraminifers. The sampling of microfossils is markedly different from macroinvertebrates, so the correspondence of patterns across these groups is unlikely to be sampling-related. In addition, we find that size reduction affected a range of ecologically and physiologically disparate clades. Evidently, the selective pressures on size ultimately resulted from either widespread environmental change or the restructuring of ecosystems on a global scale.
Not only do we find Early Triassic size reduction in several marine clades, but the size decrease is also greater than can be explained by the loss of diversity at the boundary. We expect to see a reduction in maximum size after all mass extinctions even if species extinction was random with respect to size. However, reduction in diversity alone does not account for all Early Triassic reduction in maximum size, as observed maximum sizes during Induan time remain below diversity-corrected maximum values for Late Permian stages in most clades (Fig. 3B). This analysis demonstrates that there is change in the underlying size distribution that is not just due to the changes in diversity over time. Thus, size evolution reflects additional ecological and environmental pressures beyond diversity loss.
Although many marine groups had unusually small size distributions in the earliest Triassic (Induan), they show signs of size recovery starting in the late Early Triassic (Olenekian). Previous work on gastropods indicates that small size ranges persisted through the entire Early Triassic (Fraiser and Bottjer Reference Fraiser and Bottjer2004; Payne Reference Payne2005), but here we find that most marine clades already exhibit size increase during the late Early Triassic. Size recovery beginning in the Olenekian is consistent with the comparatively large Early Triassic gastropods described by Brayard et al. (Reference Brayard, Nützel, Stephen, Bylund, Jenks and Bucher2010). In contrast, trace fossils remain small in the latest Early Triassic relative to their pre-extinction and Middle Triassic counterparts (Pruss and Bottjer Reference Pruss and Bottjer2004), suggesting that some organisms had slower size recovery than the clades examined here. The size reduction phenomenon may not have lasted as long as previously thought because recent radiometric dates have shortened the Early Triassic time scale; in particular, the Induan stage now appears to have lasted less than two million years (Ovtcharova et al. Reference Ovtcharova, Bucher, Schalteger, Galfetti, Brayard and Guex2006; Burgess et al. Reference Burgess, Bowring and Shen2014). Nevertheless, the fact that small size distributions are observed in the Induan indicates that this phenomenon endured for at least the duration of this stage. Early Triassic conditions must have favored small body size in order for this pattern of size reduction to be preserved.
Clade-Specific Size Trends
Even though size reduction is prevalent among marine clades in the Early Triassic, how size decrease is accomplished differs between taxonomic groups. Few previous studies have explicitly decomposed size change into among-lineage and within-lineage components (Rego et al. Reference Rego, Wang, Altiner and Payne2012), but here we evaluate the relative importance of size-biased extinction, size-biased origination, and within-lineage size evolution across time and taxa. Because of the relationship between large body size and small population size, one might expect extinction events to selectively eliminate larger taxa. Although some evidence points to size-selective extinction or recovery in certain taxa (Arnold et al. Reference Arnold, Parker and Hansard1995b; Lockwood Reference Lockwood2005), there has been no consistent relationship found between body size and extinction probability in the marine invertebrate fossil record (Jablonski and Raup Reference Jablonski and Raup1995; McRoberts and Newton Reference McRoberts and Newton1995; Jablonski Reference Jablonski1996; Lockwood Reference Lockwood2005). Size reduction across the Permian/Triassic boundary resulted from at least two different modes of size change: extinction of larger species and evolution of surviving lineages toward smaller sizes. This within-lineage component of size decrease cannot be explained by the end-Permian extinction mechanism. The extinction was geologically rapid, but species that became smaller retained their small size well into the Early Triassic. Observed rates of size evolution (e.g., Lister Reference Lister1989; Vartanyan et al. Reference Vartanyan, Garutt and Sher1993; Gingerich Reference Gingerich2009) would allow for very rapid size recovery relative to our temporal resolution. Therefore, Early Triassic environmental conditions or ecological pressures continued to favor small body size.
Although most marine clades show size decrease in the earliest Triassic, those that behave differently can shed light on the processes controlling size reduction and recovery. Ammonoids stand out as the exception to the pattern of size decrease at the Permian/Triassic boundary. Whereas other clades decreased in median size across the boundary, ammonoids increased significantly, and they showed little change in maximum size while other groups lost all of their largest species. Most marine clades are near their smallest median sizes in the Induan, but ammonoid median size is large compared to the rest of their Permian-Triassic size history. Perhaps with finer time resolution, one could resolve a size decrease in ammonoids as well, but even if so, they certainly recovered faster than any other group studied. Ammonoids are also unusual in that they showed rapid recovery in diversity after the end-Permian extinction compared with benthic groups like the gastropods and bivalves (Brayard et al. Reference Brayard, Escarguel, Buchner, Monnet, Brühwiler, Goudemand, Galfetti and Guex2009). The appearance of larger ammonoid species is likely related to this rapid recovery.
When comparing the skeletal physiology, life habit, motility, trophic level, and other traits of our eight marine clades, the ammonoids are distinguished by their nektonic habitat. The other nektonic clade in our dataset, the conodonts, decrease in median size at the Permian/Triassic boundary but show similarly large size changes in nearly all other stages as well. Neither clade decreases substantially in maximum size in the earliest Triassic. Nektonic mode of life may have afforded release from the selective pressures driving size reduction.
Controls on Size Evolution
In general, evolutionary size change may result from changes in the abiotic or biotic environment. Previous work has highlighted three possible selective pressures in order to explain the small sizes of Early Triassic marine organisms: (1) physical environmental constraints (e.g., hypoxia) (Fraiser and Bottjer Reference Fraiser and Bottjer2004; Twitchett Reference Twitchett2007; Song et al. Reference Song, Tong and Chen2011), (2) low food availability (Twitchett Reference Twitchett2001; He et al. Reference He, Twitchett, Zhang, Shi, Feng, Yu, Wu and Peng2010), and (3) low predation or competition pressure (Payne Reference Payne2005). The end-Permian and Early Triassic geologic record is rife with evidence of potential environmental constraints on maximum size. The interval is characterized by persistent or reoccurring toxic ocean waters, including shallow marine anoxia, hypercapnia, sulfidic conditions, or a combination of toxins (Hallam Reference Hallam1991; Isozaki Reference Isozaki1997; Wignall and Twitchett Reference Wignall and Twitchett2002; Grice et al. Reference Grice, Cao, Love, Bottcher, Twitchett, Grosjean, Summons, Turgeon, Dunning and Jin2005; Kump et al. Reference Kump, Pavlov and Arthur2005; Knoll et al. Reference Knoll, Bambach, Payne, Pruss and Fischer2007). In modern oceans, the body size of marine organisms decreases as oxygen concentration decreases (Levin Reference Levin2003; Gooday et al. Reference Gooday, Levin, Aranda da Silva, Bett, Cowie, Dissard, Gage, Hughes, Jeffreys, Lamont, Larkin, Murty, Schumacher, Whitcraft and Woulds2009), so we expect to see a similar pattern in ancient environments. If hypoxia was a problem for end-Permian and Early Triassic marine communities, seafloor waters would have less chance of mixing with atmospheric oxygen and benthic clades might have been particularly susceptible. On the other hand, free movement within the water column may have afforded ammonoids the opportunity to escape unfavorable environmental conditions at different water depths or in localized geographic areas. In addition to their nektonic habitat, ammonoids may have had low sensitivity to hypoxia like some of their extant cephalopod relatives (for example, vampire squid and nautilus) (Seibel et al. Reference Seibel, Chausson, Lallier, Zal and Childress1999; Marshall and Jacobs Reference Marshall and Jacobs2009). The ability to escape or thrive in low oxygen conditions may have been important for the evolution of large size in the Early Triassic.
Furthermore, the magnitude of size decrease in a marine clade may relate to their sensitivity to changes in ocean chemistry. Knoll et al. (Reference Knoll, Bambach, Payne, Pruss and Fischer2007) found that groups lacking respiratory and circulatory systems and secreting proportionally massive calcareous skeletons suffered greatly elevated extinction rates at the end-Permian. They argue that hypercapnic stress from elevated pCO2 best explains this extinction selectivity. Similarly, the clades with the least potential for physiological buffering against change in ambient environmental conditions, calcitic brachiopods and foraminiferans, show the largest decreases in both median and maximum size across the extinction horizon. In contrast, the clades with the smallest changes in maximum size (ammonoids and conodonts) were likely to have been better buffered against changes in ocean chemistry due to their ability to use gills and closed circulatory systems to buffer their internal chemistry relative to change in seawater and their ability to precipitate their skeletons from physiologically well buffered fluids (Knoll et al. Reference Knoll, Bambach, Payne, Pruss and Fischer2007).
Another possible cause of Early Triassic size reduction is food shortage due to primary productivity decline (Twitchett Reference Twitchett2001; He et al. Reference He, Twitchett, Zhang, Shi, Feng, Yu, Wu and Peng2010). However, at least some clades of predatory organisms (ammonoids and conodonts) were less affected by the extinction, suggesting that there was sufficient primary productivity to maintain diverse and large-bodied organisms at high trophic levels. In addition, if the Early Triassic was a time of decreased export productivity, we would expect to find reduction of the carbon isotope gradient between shallow and deep water, as is observed after the end-Cretaceous mass extinction (Arthur et al. Reference Arthur, Zachos and Jones1987; D’Hondt et al. Reference D’Hondt, Donaghay, Zachos, Luttenburg and Lindinger1998). Instead, there is evidence for a large δ13C gradient with water depth (Meyer et al. Reference Meyer, Yu, Jost, Kelley and Payne2011; Song et al. Reference Song, Tong, Algeo, Horacek, Qiu, Song, Tian and Chen2013), consistent with high primary productivity and anoxic and sulfidic conditions in the water column. Geochemical models suggest that prolonged ocean anoxia, such as proposed during this time, requires high rates of primary production (Meyer et al. Reference Meyer, Kump and Ridgwell2008; Ozaki et al. Reference Ozaki, Tajima and Tajika2011). Increased bacterial productivity after the end-Permian extinction (Xie et al. Reference Xie, Pancost, Jin, Wang and Evershed2005) may have lowered the quality of food resources for marine animals (Payne and Finnegan Reference Payne and Finnegan2006). However, the primary productivity decline scenario does not appear to be consistent with evidence for extensive hypoxia during the Early Triassic.
Finally, the correlation between size reduction and mass extinctions suggests there may be a direct link between biodiversity and selective pressures on size. There is evidence from a few clades for size decrease at other extinction events, including the end-Ordovician (Holland and Copper Reference Holland and Copper2008; Huang et al. Reference Huang, Harper, Zhan and Rong2010; Borths and Ausich Reference Borths and Ausich2011; Baarli Reference Baarli2014), Frasnian/Famennian (Renaud and Girard Reference Renaud and Girard1999; Balinski Reference Balinski2002), end-Triassic (Végh-Neubrandt Reference Végh-Neubrandt1982), Pliensbachian/Toarcian (Morten and Twitchett Reference Morten and Twitchett2009), and end-Cretaceous (Arnold et al. Reference Arnold, Kelly and Parker1995; Smith and Jeffery Reference Smith and Jeffery1998; Lockwood Reference Lockwood2005). There is also some evidence that maximum body size tracks diversity history more generally in bivalves, cetaceans, and crinoids (Trammer Reference Trammer2005). The loss of taxonomic diversity may favor small size by reducing predation pressure and competition among survivors. Reduced defensive ornamentation and rates of shell crushing and drilling indicate decreased predation pressure in the Early Triassic (Boyd and Newell Reference Boyd and Newell1972; Valentine Reference Valentine1973; Kowalewski et al. Reference Kowalewski, Dulai and Fürsich1998). Therefore, to the extent that large size represents a refuge from predation (e.g., Paine Reference Paine1976; Harper et al. Reference Harper, Peck and Hendry2009), there would be less selection against small individuals after a major extinction event. In addition, the low diversity of Early Triassic communities may have limited competitive interactions, and thus the competitive displacement of size (Brown and Wilson Reference Brown and Wilson1956; Hutchinson Reference Hutchinson1959). Further supporting the link between diversity and size, the clades that exhibit more rapid diversification in the Early Triassic (ammonoids and conodonts) (Orchard Reference Orchard2007; Brayard et al. Reference Brayard, Escarguel, Buchner, Monnet, Brühwiler, Goudemand, Galfetti and Guex2009) also show little change in maximum size across the Permian/Triassic boundary.
The size-evolution patterns in the eight marine clades we examined here are consistent with both scenarios of physical environmental stress and reduced competition or predation pressure. However, given the differences in how size change is accomplished among taxonomic groups, it may be inappropriate to look for a single mechanistic cause for the Lilliput Effect. Size-biased extinction was likely linked to the end-Permian extinction mechanism, whereas within-lineage evolution towards smaller size reflects the abiotic and/or biotic environment of the Early Triassic. The relative importance of among-lineage and within-lineage processes of size change varies from clade to clade during the size recovery as well. In addition, though most higher taxa exhibit Early Triassic size reduction, the magnitude of size decrease differs between clades. Although the end-Permian mass extinction was almost certainly the ultimate trigger for Early Triassic size reduction, these different patterns and modes of size change among clades indicate the proximal causes may be more complex. Some clades may respond more strongly to selection pressures from competition and predation, while others are more sensitive to dissolved oxygen concentration, pCO2, pH, carbonate saturation, or a combination of factors. All of these proximal causes were likely at work in the Early Triassic, and it may prove difficult to isolate which were acting on which groups of organisms. Our understanding of clade-specific controls on size evolution should improve with the comparison of size dynamics across multiple clades through time.
Summary
Quantifying patterns of size evolution in eight well-fossilized marine clades across the end-Permian extinction and recovery reveals changes in the size distribution of these taxa on a global scale as well as differences in size dynamics between clades. Size reduction after the end-Permian extinction is a real phenomenon for most higher taxa, but does not last through the whole Early Triassic: unusually small size distributions in the earliest Triassic (Induan) are followed by size recovery in the late Early Triassic and Middle Triassic. Interestingly, the decrease in maximum species size at the extinction horizon is greater than expected from the loss of diversity. Calculating the relative contributions of among- and within-lineage components of size change shows that in some clades, Early Triassic size reduction results from size-selective extinction, whereas in other clades, the surviving species evolve toward smaller size. This within-lineage component of size reduction suggests that the end-Permian and perhaps other mass extinctions not only influence size evolution by selecting against larger organisms; in their aftermath, mass extinctions also create environmental or ecological pressures that particularly favor small size. Although the relative importance of environmental and biological selective pressures favoring small size remains unclear, the different size behavior of ammonoids suggests a couple possible interpretations. High evolutionary rates and rapid diversity recovery in Early Triassic ammonoids may have enhanced size displacement through increased competition and predation pressure. Alternatively, nektonic habitat or greater physiological buffering capacity may have allowed this clade to attain both Early Triassic size increase and rapid diversification in contrast to size decrease and slow recovery in benthic clades. The ultimate cause of the Early Triassic size reduction appears to have been the end-Permian environmental and biotic crisis, but different patterns and modes of size decrease among clades point to clade-specific proximal controls on size change.
Acknowledgments
The authors thank A. Bachan, S. Finnegan, P. Harnik, N. Heim, A. Jost, C. Keating-Bitonti, B. Kelley, K. Lau, and K. Meyer for comments and discussion, and N. Nogales Lopez and K. Vanderboll for data collection. This work was supported by the U.S. National Science Foundation (EAR-1151022), the Shell Foundation, and Stanford University (Bio-X Interdisciplinary Initiative Program).