Introduction
Genomic imprinting relates to the field of epigenetics where maternal or paternal alleles are fully or partially inactivated. Imprinting effects belong to the group of parent-of-origin effects (POEs) as they arise due to DNA-modifications taking place during each gametogenesis depending on the sex of an animal. An example of the relevance of POEs in livestock is a maternally imprinted quantitative trait locus (QTL) in the IGF2 region in pig showing a large effect on muscle mass and fat deposition (e.g. Nezer et al., Reference Nezer, Moreau, Brouwers, Coppieters, Detilleux, Hanset, Karim, Kvasz, Leroy and Georges1999). Whereas this imprinted QTL was found applying a QTL mapping experiment, expression studies and variance components analyses constitute further strategies to investigate genomic imprinting. With respect to the latter, Neugebauer et al. (Reference Neugebauer, Luther and Reinsch2010a and Reference Neugebauer, Räder, Schild, Zimmer and Reinsch2010b) proposed a model (imprinting model) with two correlated parental transmitting abilities (TAs): the first accounts for the expression of genes under a paternal expression pattern, the second for the expression of genes under a maternal expression pattern. They applied their model in a reduced version (Quaas and Pollak, Reference Quaas and Pollak1980), which allowed an imprinting analysis of slaughter traits in Simmental, a breed for which large data sets are available.
Our objective was to analyse four value-determining slaughter traits of 1 366 160 fattening bulls accompanied by pedigrees of up to 2 637 761 Simmental ancestors to investigate the relative imprinting variances. The size of the data set generated an equation system which was still too large to be solved, even when the reduced imprinting model was used. Therefore, we adapted a parsimonious imprinting model that only contained paternal effects where the TAs as maternal grandsire (MGS) replaced the TAs as dam. This further reduced equations and enabled the inclusion of all data. Moreover, an equivalent model Blunk et al. (Reference Blunk, Mayer, Hamann and Reinsch2017) allowed the direct estimation of POEs together with their prediction error variances (PEVs).
Material and methods
Pedigree and slaughter house data
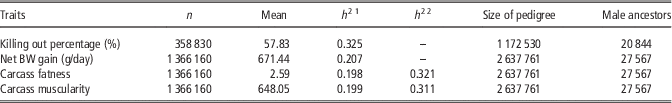
Within the scope of progeny field tests from 1995 to 2014, slaughter data of Austrian and German Simmental fattening bulls were collected. The genetic evaluation centre of the Landesamt für Geoinformation und Landentwicklung (LGL) in Baden-Württemberg, Germany, provided data of four slaughter traits routinely recorded by 62 abattoirs. Killing out percentage (i.e. carcass weight divided by live weight, %) was available for 358 830 animals after editing. Net BW gain (carcass weight divided by age, g/day), carcass fatness and carcass muscularity were available for 1 366 160 animals. Carcass fatness was defined using classes from 1 (very lean) to 5 (very fat). Carcass muscularity was treated in accordance to the E-U-R-O-P system (E=excellent to P=poor), which was replaced by monetary values (670, 655, 635, 585, 525). The pedigrees contained up to 2 637 761 ancestors (Table 1).
Number of fattening bulls (n), mean, heritability (h 2), size of the pedigree and the number of male ancestors for all traits

1 Linear model with a sire effect assuming no imprinting. The SE were below 0.009.
2 Generalised linear model with a sire effect assuming no imprinting. The SE were below 0.007.
The parsimonious model
When genomic imprinting exists, the two parental TAs of the imprinting model are different and the variation of this difference refers to the imprinting variance. In a reduced version of the model, the two TAs are only fitted for ancestors which reduces the number of equations to be solved. Nonetheless, the data set used in this study was still too large to estimate the genetic parameters. Therefore, we replaced the TAs as dam within the imprinting model by the corresponding TAs as MGS reflecting the maternal side of expression. As genetic parameters were then only predicted for male ancestors, 20 844 ancestors remained for killing out percentage and 27 567 for net BW gain, carcass fatness and carcass muscularity. The parsimonious model is:
 $$y{\bf \,=\,}X\bibeta {\bf {\plus}}Z_{s} a_{s} {\bf {\plus}}Z_{{mgs}} a_{{mgs}} {\plus}e,$$
where y is equal to the phenotype; β is a vector of fixed effects; a s and a mgs are vectors of TAs as sire and TAs as MGS; e the random residual; and X , Z s and Z mgs are incidence matrices connecting the effects to their observations. The variance components of the genetic effects in terms of gametic variances following Neugebauer et al. (Reference Neugebauer, Luther and Reinsch2010a and Reference Neugebauer, Räder, Schild, Zimmer and Reinsch2010b) are:
 $${\rm Var}\left[ {\matrix{ {a_{s} } \cr {a_{{mgs}} } \cr } } \right]=\left[ {\matrix{ {{1 \mathord{\left/ {\vphantom {1 2}} \right. \kern-\nulldelimiterspace} 2}A\bisigma _{s}^{2} } & {{1 \mathord{\left/ {\vphantom {1 2}} \right. \kern-\nulldelimiterspace} 2}\left( {{1 \mathord{\left/ {\vphantom {1 2}} \right. \kern-\nulldelimiterspace} 2}A\bisigma _{{sd}} } \right)} \cr {{1 \mathord{\left/ {\vphantom {1 2}} \right. \kern-\nulldelimiterspace} 2}\left( {{1 \mathord{\left/ {\vphantom {1 2}} \right. \kern-\nulldelimiterspace} 2}A\bisigma _{{sd}} } \right)} & {{1 \mathord{\left/ {\vphantom {1 4}} \right. \kern-\nulldelimiterspace} 4}\left( {{1 \mathord{\left/ {\vphantom {1 2}} \right. \kern-\nulldelimiterspace} 2} {\bi A}\bisigma _{d}^{2} } \right)} \cr } } \right]$$
where the variance
 ${1 \mathord{\left/ {\vphantom {1 2}} \right. \kern-\nulldelimiterspace} 2}\sigma _{d}^{2} $
is the variance of the TAs as dam in the imprinting model and 1/2σ
sd
the covariance between
 ${1 \mathord{\left/ {\vphantom {1 2}} \right. \kern-\nulldelimiterspace} 2}\sigma _{s}^{2} $
and
 ${1 \mathord{\left/ {\vphantom {1 2}} \right. \kern-\nulldelimiterspace} 2}\sigma _{d}^{2} $
. The mixed model equations are:
 $$\eqalignno{ &\left[ {\matrix{ {X^{'} W^{{{\minus}1}} X} & {X^{'} W^{{{\minus}1}} Z_{s} } & {X^{'} W^{{{\minus}1}} Z_{{mgs}} } \cr {Z_{s}^{'} W^{{{\minus}1}} X} & {Z_{s}^{'} W^{{{\minus}1}} Z_{s} {\plus}A^{{{\minus}1}} \lambda _{1} } & {Z_{s}^{'} W^{{{\minus}1}} Z_{{mgs}} {\plus}A^{{{\minus}1}} \lambda _{2} } \cr {Z_{{mgs}}^{'} W^{{{\minus}1}} X} & {Z_{{mgs}}^{'} W^{{{\minus}1}} Z_{s} {\plus}A^{{{\minus}1}} \lambda _{2} } & {Z_{{mgs}}^{'} W^{{{\minus}1}} Z_{{mgs}} {\plus}A^{{{\minus}1}} \lambda _{3} } \cr } }\right] \cr&\quad \left[ {\matrix{ \bibeta \cr {a_{s} } \cr {a_{{mgs}} } \cr } } \right]=\left[ {\matrix{ {X^{'} W^{{{\minus}1}} y} \cr {Z_{s}^{'} W^{{{\minus}1}} y} \cr {Z_{{mgs}}^{'} W^{{{\minus}1}} y} \cr } } \right]$$
where A contains the additive genetic relationships between sires and MGS and λ is:
 $$\left[ {\matrix{ {\lambda _{1} } & {\lambda _{2} } \cr {\lambda _{2} } & {\lambda _{3} } \cr } } \right]^{{{\minus}1}} ={1 \over {2\sigma _{R}^{2} }}\left[ {\matrix{ {\sigma _{s}^{2} } & {{1 \mathord{\left/ {\vphantom {1 2}} \right. \kern-\nulldelimiterspace} 2}\sigma _{{sd}} } \cr {{1 \mathord{\left/ {\vphantom {1 2}} \right. \kern-\nulldelimiterspace} 2}\sigma _{{sd}} } & {{1 \mathord{\left/ {\vphantom {1 4}} \right. \kern-\nulldelimiterspace} 4}\sigma _{d}^{2} } \cr } } \right]$$
where
 $\sigma _{R}^{2} $
is the residual variance in a reduced model. The diagonal matrix
W
adjusts the variation of residuals to the variation of Mendelian sampling due to the parental inbreeding coefficients
F
s
and
F
mgs
has the diagonal elements:
 $$w_{{ii}} =\left[ {{{\sigma _{R}^{2} \,{\minus}\,{1 \mathord{\left/ {\vphantom {1 2}} \right. \kern-\nulldelimiterspace} 2}F_{{s_{i} }} \sigma _{s}^{2} \,{\minus}\,{1 \mathord{\left/ {\vphantom {1 8}} \right. \kern-\nulldelimiterspace} 8}F_{{mgs_{i} }} \sigma _{d}^{2} } \over {\sigma _{R}^{2} }}} \right]^{\!{{\minus}1}} $$
In accordance with Neugebauer et al. (Reference Neugebauer, Luther and Reinsch2010a and Reference Neugebauer, Räder, Schild, Zimmer and Reinsch2010b) the imprinting variance is
 $\sigma _{i}^{2} =\sigma _{s}^{2} {\plus}\sigma _{d}^{2} \,{\minus}\,2\sigma _{{sd}} $
and the additive genetic variance is
 $\sigma _{a}^{2} =\sigma _{s}^{2} {\plus}\sigma _{d}^{2} $
.
The significance of the imprinting variances was statistically verified using a REML likelihood ratio test with two degrees of freedom (Neugebauer et al., Reference Neugebauer, Luther and Reinsch2010a and Reference Neugebauer, Räder, Schild, Zimmer and Reinsch2010b). Whereas the alternative hypothesis (i.e. existence of imprinting) was presented by fitting the parsimonious model, the null hypothesis (non-existence of imprinting) was presented by fitting an equivalent model with one genetic effect as sire.
In case the imprinting variance turned out to be significant, the POEs were directly delivered as the deviation from the TAs as sire using an equivalent parsimonious model. Their PEVs could be easily derived from the diagonal elements of the inverted coefficient matrix and were used to calculate the reliabilities with
 $r^{2} =1{\minus}{{PEV} \mathord{\left/ {\vphantom {{PEV} \sigma _{i}^{2} }}} \right. \kern-\nulldelimiterspace} {1 \mathord{\left/ {\vphantom {1 8}} \right. \kern-\nulldelimiterspace} 8}\,{\sigma_{i}^{2}(1{\plus}{F_i)}}$
where Fi is the inbreeding coefficient of an animal i. The genetic parameters were derived via the ASReml-package (Gilmour et al., Reference Gilmour, Gogel, Cullis and Thompson2009).
Model effects
The estimation of genetic parameters based on the following model effects:
 $$\eqalignno{ y_{{ijklmn}} = BS_{i} &{\plus} KN_{j} {\plus} GT_{k} {\plus} b_{1} x {\plus} b_{2} x^{2} {\plus} b_{3} x^{3} \cr&\!\!\!\!\!\!\!\!\! {\plus} a_{{s_{l} }} {\plus} a_{{mgs_{m} }} {\plus} e_{{ijklmn}}, $$
where y
ijklmn
defines the beef traits; BS
i
the fixed effect of the interaction of farm and slaughter date; KN
j
and GT
k
the fixed effects of parity number and birth type; b corresponds to the linear (b
1), quadratic (b
2) and cubic (b
3) regression on slaughter age x;
 $a_{{s_{l} }} $
the TA of sire l;
 $a_{{mgs_{m} }} $
the TA of MGS m; and e
ijlkmn
the random residual. Furthermore, fat class and carcass muscularity were assumed to be binomially distributed and analysed using a GLM with a logit-link function.
Results and discussion
Significance of imprinting variances and parental contributions
Significant imprinting variances were found for all analysed traits (P-values <0.001). The relative imprinting variances
 $\left( {{{\sigma _{i}^{2} } \mathord{\left/ {\vphantom {{\sigma _{i}^{2} } {\sigma _{a}^{2} }}} \right. \kern-\nulldelimiterspace} {\sigma _{a}^{2} }}} \right)$
were 14.15% for killing out percentage, 12.41% for net BW gain, 16.64% (GLM: 17.13%) for carcass fatness and 8.56% (GLM: 10.31%) for carcass muscularity. The result for killing out percentage confirmed findings of Neugebauer et al. (Reference Neugebauer, Räder, Schild, Zimmer and Reinsch2010b) who reported a relative imprinting variance of 24.56% in German Simmental. In contrast, they could not detect a significant imprinting variance in net BW gain. With regard to carcass fatness, Engellandt and Tier (Reference Engellandt and Tier2002) provided evidence for the existence of POEs on fat traits in German Gelbvieh cattle. With regard to carcass muscularity, our findings agree with those reported by Neugebauer et al. (Reference Neugebauer, Räder, Schild, Zimmer and Reinsch2010b) with 10.75%.
The paternal contribution to the imprinting variance was calculated with
 $\left( {\sigma _{s}^{2} {\minus}\sigma _{{s,d}} } \right)/\sigma _{i}^{2} $
and the maternal contribution with
 $\left( {\sigma _{d}^{2} {\minus}\sigma _{{s,d}} } \right)/\sigma _{i}^{2} $
. The imprinting variances in killing out percentage, net BW gain and carcass muscularity were mainly constituted by maternal gametes with 70.07%, 82.20% and 62.94% (GLM: 82.36%). The imprinting variance for carcass fatness almost equally consisted of both parental variances.
It needs to be borne in mind that some factors can generally not be considered using the parsimonious model as they are solely inherited by females and must thus be considered as nuisance factors possibly inflating the imprinting variance. A non-negligible factor might be the X-chromosome which is, for example, responsible for 5% to 10% of the genetic variation for milk production following VanRaden (Reference VanRaden1987). The predicted effects should thus not be referred to as imprinting effects but as the more general term of POEs.
Heritabilities
We first applied the model without POEs to estimate the heritabilities (h 2) summarised in Table 1. The heritability estimates were 0.33 for killing out percentage, 0.21 for net BW gain and 0.20 for fat score (GLM: h 2=0.32) and carcass muscularity (GLM: h 2=0.31). The heritability estimate for killing out percentage exceeds the finding of Neugebauer et al. (Reference Neugebauer, Räder, Schild, Zimmer and Reinsch2010b) who estimated a h 2 of 0.22 in German Simmental using an animal model without POEs. In contrast, their estimates for net BW gain (h 2=0.28), carcass fatness (h 2=0.25) and carcass muscularity (h 2=0.31) were higher than our findings. With regard to the latter two traits, deviating results may, however, be due to different carcass quality trait definitions as Neugebauer et al. (Reference Neugebauer, Räder, Schild, Zimmer and Reinsch2010b) used 15 video-recorded categories.
Using the parsimonious model led to heritability estimates of 0.37 for killing out percentage, 0.23 for net BW gain, 0.21 (GLM: h 2=0.35) for carcass fatness and 0.21 (GLM: h 2=0.35) for carcass muscularity. In comparison to the h 2 estimated using the model without POEs, a slight increase may be explained by the additional consideration of genetic information due to the incorporation of the MGS effect in the model. The reason is that, as shown earlier, the maternal gamete contributes more to the genetic variance, which is not accounted for by using the model containing only one genetic effect as sire (i.e. without POEs).
Reliabilities of parent-of-origin effects
The average reliabilities of POEs (which were calculated using the equivalent parsimonious model) Blunk et al. (Reference Blunk, Mayer, Hamann and Reinsch2017) were 0.20 for killing out percentage, 0.18 for net BW gain, 0.19 for carcass fatness and 0.16 for carcass muscularity. The GLM led to identical results for carcass fatness. For carcass muscularity the GLM yielded an average reliability of 0.17. Considering the reliabilities of POEs on a time-scale from 1950 to 2010, an increase in reliabilities became visible since the mid-1960s and achieved a maximum for animals born between 1980 and 1995. This might be due to improved data collection during these years as reliabilities are mainly dependent on the data availability. As the model used in this study includes two genetic effects, many records of sons as well as of maternal grandsons are needed to achieve reliable effects. An examination of data confirms these conditions: whereas animals possessing POEs with reliabilities <0.4 have an average number of 15 sons and 16 maternal grandsons with records, animals possessing POEs with reliabilities >0.4 have an average number of 993 sons and 978 maternal grandsons with records.
Conclusion
The parsimonious model, reflecting both parental expression patterns by incorporating a sire and MGS effect, allowed the exploitation of large data and indicated significant contributions of POEs to the additive genetic variance in beef traits in dual-purpose Simmental.
Acknowledgements
The authors gratefully acknowledge financial support from the H. Wilhelm Schaumann-Stiftung, Hamburg.