Introduction
A high-energy and high-protein diet is generally fed to weaning rabbits. Soya-bean meal (SBM) and groundnut meal are important protein sources that are conventionally added in rabbit diets. However, these protein sources are also included in human diet and due to increasing human population in Asian subcontinents there is a need to find alternate protein sources for rabbits. Animal production in tropical countries is largely based on alternate feed resources that did not compete with human foods. Economisation of feed cost using cheaper and unconventional feed resources (Vasanthakumar et al., Reference Vasanthakumar, Sharma, Sastry and Kumar1999; Bhatt and Sharma, Reference Bhatt and Sharma2001; Muriu et al., Reference Muriu, Njoka-Njiru, Tuitoek and Nanua2002) is an important aspect of commercial rabbit production. India is the second largest producer of rapeseed (Brassica napus)-mustard (Brassica juncea) in the world and produces one-fifth of the world’s total rapeseed-mustard (Kiresur, 1999). Mustard meal (MM) is a by-product of oil extraction industries and it contains 300 to 395 g crude protein (CP) per kg MM on dry-matter (DM) basis (Tripathi and Singhal, 1994). The MM is also rich in sulphur, with the content ranging from 14.3 to 23.0 g/kg MM (Papas et al., Reference Papas, Ingalls and Cansfield1978; Tyagi et al., Reference Tyagi, Tripathi and Karim1996). In spite of its well-balanced amino acid composition (Pastuszewska et al., Reference Pastuszewska, Jablecki, Swiich, Buraczewska and Ochtabinska2000), the use of MM in rabbit feeding is limited mainly because of the high content of glucosinolates. The glucosinolate content of MM made from Indian mustard varieties ranges between 12 and 90 mg/g meal (Chauhan et al., Reference Chauhan, Jha, Yadav, Kumar, Shukla and Singh1999). Glucosinolates are non-toxic, but upon degradation thiocyanate, isothiocyanates and nitriles are released that are toxic to animals. These end products suppress the thyroidal uptake of iodine (Duncan, Reference Duncan1991; Barrett et al., Reference Barrett, Klopfenstein and Leipold1997) and induce metabolic disorders such as liver and thyroid hypertrophy (Papas et al., Reference Papas, Ingalls and Campbell1979; Fenwick and Curtis, Reference Fenwick and Curtis1980; Bourdon et al., Reference Bourdon, Perez and Baudet1981; Bell, Reference Bell1984). Upon ingestion, glucosinolate or metabolites may cause tissue alterations, and growth and health problems (Wallig et al., Reference Wallig, Kore, Crawshaw and Jeffery1992; Kloss et al., Reference Kloss, Jeffery, Wallig, Tumblenson and Parsons1994; Tripathi and Mishra, Reference Tripathi and Mishra2007). Adverse effect on growing broilers fed 50 to 100 g crambe meal (Ledoux et al., Reference Ledoux, Belyea, Walling and Tumbleson1999), high mortality in rat fed 100 g crambe meal per kg diet (Tookey et al., Reference Tookey, Van-Etten and Daxenbichler1980) and poor performance of pigs fed 150 g crambe meal per kg were reported (Schone et al., Reference Schone, Leiterer, Hartung, Jahreis and Tischendorf2001). Information on uses of rapeseed/crambe meal in rabbit feed is scant.
Therefore, the aim of the present study was to assess the effect of adding high-glucosinolate MM as a substitute for conventional SBM on the growth performance, caecal fermentation and concentration of blood metabolites in growing rabbits.
Material and methods
Animals and location of the study
Forty weaning rabbits (4 weeks old, 314 ± 24 g live weight (LW)) of Soviet Chinchilla and White Giant breed were used. The animals were housed in individual cages (45 cm × 50 cm × 37 cm) with the provision of food and water, which were kept inside a covered shed with a concrete floor. The house was designed to ensure cross-ventilation and to prevent rodents and other pests.
The study was carried out at the Central Sheep and Wool Research Institute, Avikanagar, located at 26° 17′N latitude, 75° 28′E longitude and 320 m above sea level. The climate is typically semi-arid with yearly mean minimum and maximum temperatures of 6°C and 41°C, respectively. The ambient temperature and relative humidity in the animal shed during the experimental period ranged between 9°C and 30°C and between 43% and 80%, respectively.
Diets and feeding management
Four complete isonitrogenous pelleted diets using ground ingredients were prepared (Table 1) at the Feed Technology Unit of the institute. The diets contained MM at 80, 160 and 245 g/kg DM. The control diet (MM 0) had SBM as the major source of protein. The weighed feed ingredients were moistened with water to achieve 25% to 30% moisture and were thoroughly mixed. The feed mixtures were then pelleted in a horizontal mini-pelleting machine. The pellets were then sun dried. There was ad libitum feeding during the experimental period (8 weeks). The diets were offered at 10:00 h daily with an allowance of 10% more than the previous day’s consumption. The feed refusal were weighed and discarded before offering fresh feed to determine the intake for the previous day. The rabbits had free access to clean drinking water. Daily records of feed intake were maintained throughout the experiment. The animals were weighed at weekly intervals.
Ingredients and chemical composition of dietsFootnote †

† Experimental diet containing 0, 80, 160 or 245 g mustard meal (MM) per kg dry matter (DM). SBM = soya-bean meal.
‡ Mixture containing (in g/kg) calcium, 320, phosphorus, 62, manganese, 2.7, zinc, 2.6; (in p.p.m.) iron, 1000, fluorine, 900, iodine, 100, copper, 100; and (in g/kg) thiamin, 0.25, riboflavin, 1.5, calcium pantothenate, 5.0, pyridoxin, 0.1, nicotinic acid, 12.5, cholcalciferol, 1, α-tocohperols, 15, cynocobalamine, 0.006 and choline chloride, 100.
§ Mean of three determinations.
¶ ND = not determined.
A metabolism trial was carried out, which was started at 56 days of age and finished on 64 days of age. Six animals of similar LW were randomly taken from each treatment and placed in metabolic cages with the facility for separate quantitative collection of urine and faeces. During the collection period of 5 days, the total voided faeces was weighed and dried in a forced draught oven at 60°C until constant weight is reached. The dried faeces samples for each animal were pooled and ground to pass a 1 mm sieve and preserved for further analysis. Voided urine was collected in acidified containers, measured and washed with distilled water everyday. Collected urine was washed well and 1% aliquot was preserved in sulphuric acid for nitrogen (N) estimation.
Caecal digesta sampling and blood collection
Caecal digesta samples were collected by slaughtering four animals from each group at 1400 h after cervical dislocation and deskining. The total digestive tract was removed by severing the middle line of the stomach, and the caecum was separated and weighed. The sample of caecum digesta was collected in wide-mouth 200 ml plastic bottles by gentle squeezing. The empty caecum was then cleaned with water flushing and weighed. A total of 10 g of caecal content was added into the Kjeldahl flask containing 25 ml of concentrated sulphuric acid for total nitrogen estimation. Another 10 g of caecal content was diluted with 15 ml of distilled water, pH was determined immediately and the contents were then filtered through four layers of muslin cloth. The sampling for NH3-N and total volatile fatty acids (TVFA) estimation was done as per the procedures of Garcia et al. (Reference Garcia, Villamide and De Blas1996), 10 g caecal content was acidified with 10 ml of 0.2 mol/l HCl and centrifuged at 5000 r.p.m. for 15 min and the supernatant was used for NH3-N. A separate 20 g caecal content was preserved with 2 ml of solution containing 5% orthophosphoric acid (v/v) and 1% HgCl2 (w/v) in equal quantities. The preserved samples were later diluted with 20 ml distilled water and centrifuged at 5000 r.p.m. for 15 min for feed particle separation and the supernatant was used for estimating total-N and microbial nitrogen by trichloroacetic acid-precipitable nitrogen (TCAppt-N) and TVFA estimations. Blood samples were collected before slaughter through ear vein puncture into heparinised serum tubes.
Chemical analysis
The pooled representative samples of SBM, MM, experimental diets, faeces, urine and muscles were analysed for chemical constituents according to standard methods of Association of Official Analytical Chemists (2000). DM was determined by drying at 80°C for 24 h (Method 934.01); CP, by using nitrogen (CP = N×6.25; method 976.05); fat (EE), by Soxhlet extraction using petroleum ether (method 920.39); and ash content by ashing in muffle furnace at 500°C for 24 h (Method 942.05). The neutral-detergent fibre (NDF) was determined using sodium sulphite and sodium lauryl sulphate as described by Van Soest et al. (Reference Van Soest, Robertson and Lewis1991). Alpha amylase was not used to determine NDF. Acid-detergent fibre (ADF) and acid-detergent lignin (ADL) were determined following the procedures as described by Goering and Van Soest, Reference Goering and Van Soest1970. NDF and ADF were expressed with residual ash. TVFA were estimated by the distillation method (Barnett and Reid, Reference Barnett and Reid1957), and NH3-N by Conway’s diffusion cell method (Conway, Reference Conway1962). The total glucosinolate (TGLS) content of the MM and experimental diets was determined using the method of Tholen et al. (Reference Tholen, Shifeng and Truscott1989). Gross energy (GE) content was determined by the Ballistic bomb calorimeter (Gallenkamp, Loughborough, UK), while metabolisable energy (ME) was calculated using the following equation (Bolis et al., 1996):

where ME is expressed in kJ/day, DE is the digestible energy in kJ/day and Nu is the nitrogen content of urine in g/day.
Mineral contents of the diet, liver and serum were estimated as per the procedures described for atomic absorption spectrophotometry. Wet digestion of the liver and serum was performed, whereas diet minerals were extracted from ash after ignition of the samples at 500°C for 24 h. Blood samples were collected through ear vein puncture. Haemoglobin, erythrocyte sedimentation rate, packed cell volume, red blood corpuscles (RBCs) and white blood cells (WBCs) were estimated following the standard procedure (Jain, Reference Jain1986), while albumin, protein, serum activities of alkaline phosphates, aspartate transaminase (AST) and alanine transaminase (ALT) were estimated using diagnostic kits (Span Diagnostic Ltd, Surat, India).
Statistical analysis
Results were subjected to test for statistical significance using the analysis of variance procedure of SPSS base 10.0 (SPSS Inc., Chicago, IL, USA), a general linear mathematical model was used:
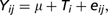
where μ is the general mean, Ti is the effect of the ith MM level (i = 1, 4) and eij is the random error. Significance among mean values of treatments was separated using Duncan’s multiple range test. Data were also subjected to polynomial design, which were tested for linear and quadratic relationship.
Results
Total glucosinolate and chemical composition
The MM used in the test diets contained 54.8 mg TGLS per g oil-extracted meal. The MM 80, MM 160 and MM 245 diets had 3.8, 8.4 and 11.98 mg TGLS per g DM, respectively (Table 1). All diets were isonitrogenous and similar in chemical constituents except for the EE content, which increased with the level of MM incorporation. The CP content of MM was lower to that of SBM. The MM-incorporated diets had lower mineral contents compared to that of the SBM diet.
Nutrient intake, coefficient of total tract apparent digestibility
The daily intake of DM in different groups during the metabolism trial period was similar, the MM incorporation influenced coefficient of total tract apparent digestibility (CTTAD) of DM and CP, and the effects were quadratic (Table 2). However, digestible protein (DP) intake and ME intake were not influenced by MM incorporation levels. The MM incorporation linearly (P < 0.05) increased the DP and ME content, and the efficiency of digestible energy to ME conversion. The DE-to-DP ratio and ME-to-DP ratio (kJ/g DP) were wider in MM-incorporated diets, which showed both linear as well as quadratic effects. The efficiency of DP (g), DE (kJ) and ME (kJ) for each g of LW gain was similar and ranged between 0.53 and 0.80 g, 47 and 66 kJ, and 46 and 65 kJ, respectively.
Nutrient intake and digestibility coefficient

a,b,cMean values in a row with different superscript letters are different at P < 0.05.
†Experimental diet containing 0, 80, 160 or 245 g mustard meal (MM) per kg dry matter.
‡NS = not significant; *P < 0.05; **P < 0.01.
§LIN = significance of linear effect of MM incorporation.
¶QUR = significance of quadratic effect of MM incorporation.
∥DE = digestible energy, DP = digestible protein; ME = metabolisable energy.
Live-weight gain
Average daily gain (ADG) reduced (P < 0.05) linearly with increasing levels of MM in diet (Table 3). Similarly, feed intake (g/day), constituents of gain and energy retained as protein and fat also depressed (P < 0.05) linearly by MM incorporation levels. DE requirement for growth and maintenance was also lower (linear, P < 0.05) for rabbits fed the MM-incorporated diet. The DE requirement (kJ/day) ranged from 1138 to 1438 for a daily gain of 26.7 to 30.7 g, and rabbits approached the marketable weight of 1.8 to 2.0 kg at the age of 12 weeks.
Average daily gain, nutrient gain and energy balance in growing rabbits

†Experimental diet containing 0, 80, 160 or 245 g mustard meal (MM) per kg dry matter.
‡NS = not significant; *P < 0.05.
§LIN = significance of linear effect of MM incorporation.
¶QUR = significance of quadratic effect of MM incorporation.
Caecum fermentation characteristics
Intestine and caecum fermentation characteristics are given in Table 4. MM incorporation linearly reduced (P < 0.05) the weight of caecum or its content, when expressed as per cent of intestine or as per cent of caecum weight, respectively. Caecum and its content as per cent of LW also reduced linearly, with increasing levels of MM in the diet.
Intestine and caecum fermentation characteristics in growing rabbits

a,b,cMean values in a row with different superscript letters are different at P < 0.05.
†Experimental diet containing 0, 80, 160 or 245 g mustard meal (MM) per kg dry matter.
‡NS = not significant; *P < 0.05; **P < 0.01.
§LIN = significance of linear effect of MM incorporation.
¶QUR = significance of quadratic effect of MM incorporation.
∥TCAppt-N = trichloroacetic acid precipitable nitrogen; TVFA = total volatile fatty acids.
The pH of the caecal content that ranged between 5.85 and 6.19 was similar among diets. Total-N content (ranged between 1.19 and 1.48 g per 100 g) and TVFA (ranged between 4.7 and 5.8 mmol per 100 g) were also similar among four diets (Table 4). However, concentration of NH3-N (mg per 100 ml) reduced linearly (P < 0.05), and ranged from 31.2 to 39.0. The concentration (mg per 100 ml) of TCAppt-N increased (linear, P < 0.01) with increasing MM levels in the diet.
Blood composition and mineral contents
Blood composition and mineral contents of the serum and liver are presented in Table 5. The effect of adding MM on blood haemoglobin, packed cell volume (PCV) and leucocyte counts was quadratic (P < 0.05), whereas total WBC counts reduced and AST activity increased linearly (P < 0.01) with increasing levels of MM. Serum protein content, erythrocyte sedimentation rate (ESR), RBC counts and activity of ALT and alkaline phosphatase activity were not influenced by MM incorporation.
Blood compositionFootnote † and mineral contents in serum and liver of growing rabbits

a,b,c Mean values in a row with different superscript letters are different at P < 0.05.
† PCV = packed cell volume; RBC = red blood cells; DLC-L = differential leucocyte count – lymphocyte; DLC-M = differential leucocyte count – monocyte; DLC-N = differential leucocyte count – neutrophil; AST = aspartate aminotransferase; ALT = alanine aminotransferase.
‡ Experimental diet containing 0, 80, 160 or 245 g mustard meal (MM) per kg dry matter.
§ NS = not significant; *P < 0.05; **P < 0.01.
¶ LIN = significance of linear effect of MM incorporation.
∥ QUR = significance of quadratic effect of MM incorporation.
The content of Zn and Mg in serum and the contents of Zn, Mn, Na and Mg in liver were similar but the concentration of Cu, Na and K increased (P < 0.05). The concentration of Cu (quadratic, P < 0.05) and K (linear, P < 0.05) in the liver reduced when MM replaced SBM in rabbit diets.
Discussion
MM contains 350 to 390 g CP per kg DM utilisation of MM in rabbit diets as protein supplement offers an opportunity to economise the cost of rabbit production. But the presence of glucosinolate in the meal limits efficient utilisation in animal feeding. More than 10 mg/kg glucosinolates is toxic to pigs and poultry (Fenwick and Curtis, Reference Fenwick and Curtis1980), and responsible for poor growth and lower thyroid hormone levels (Papas et al., Reference Papas, Ingalls and Campbell1979; Tripathi, 1999). The TGLS content of MM used in this experiment was within the normal range (Chauhan et al., Reference Chauhan, Jha, Yadav, Kumar, Shukla and Singh1999) reported for Indian rapeseed-mustard meal. Although the level of adversity on animal health and production is associated with the level of rapeseed-mustard meal in the diet and its TGLS content, neither mortality nor the adverse effect of TGLS on health and growth performance of rabbits up to 160 g MM per kg diet was observed. Contrary to the present finding, McNeill et al. (Reference McNeill, Bernard and MacLeod2004) recommended a restricted use of even 00 rapeseed meal in broiler rabbit feeding and exceeding the inclusion level by more than 10% was found to reduce the intake and growth. Possibly, the process of complete feed pelleting involves the inclusion of 30% moisture, which may favour activation of the myrosinage enzyme present in rapeseed-mustard meal and responsible for TGLS degradation (Mukherjee et al., Reference Mukherjee, Afzalpurkar and El-Nockrashy1976). Myrosinase is deactivated at a temperature of 70°C to 80°C (Gil and Macleod, Reference Gil and Macleod1980), which was observed in the pelleting chamber of the pelletiser. The TGLS degradation products that arose due to activation of the myrosinase would have evaporated during pellet processing and drying (Verkerk et al., Reference Verkerk, Gaag, Dekker and Jongen1997); thus, the TGLS content of the MM-incorporated diets was lower than that of the pre-mixes. The TGLS content of the unpelleted feed mixture was 4.4 mg/g in 80 g, 9.1 mg/g in 160 g and 13.6 mg/g DM in 245 g MM diets. Rabbits in present experiment tolerated 8 mg TGLS per g diet during the active-growth phase without any adverse effect on growth and health.
The ADG (27 to 30 g/day) of rabbits in the present study was lower than reports of temperate locations (Butcher et al., Reference Butcher, Bryant and Owens1983; Al-Bar and Al-Aghbari, 1996; Bielanski et al., 1996; De Blas et al., 1996); however, this gain is in agreement with the reports of tropical locations (Rahim et al., 1996; Aboul-Ela et al., 1996; Prasad et al., Reference Prasad, Sankhyan and Karim1998). Although the intake of DM was higher (9.5% to 10.8% of body weight) than the normal requirement (4.6% to 7.0% of body weight) of growth (Prud’hon, Reference Prud’hon1968), still DM intake and growth of rabbits fed the 245 MM diet was lower than other diets. Higher TGLS breakdown products in the 245 MM diet could have resulted in the lower feed intake, which in turn reduced the growth rate (Pusztai, Reference Pusztai1989). Anti-nutritional effects of glucosinolates in rat, mice and pig are the severe intake and growth depression. Impaired intake and growth are related to the glucosinolates content in the diet. Rat diet containing 100 g crambe meal in each kg DM resulted in poor gain and increased thyroid (Wallig et al., Reference Wallig, Belyea and Tumbleson2002). Glucosinolates-associated deleterious effects are due to change in thyroid morphology, resulting in irregular follicle size, decreased colloid and sloughing of follicular cells; however this glucosinolate level did not affect blood parameters (Aumaitre et al., Reference Aumaitre, Bourdon, Peiniau and Freire1989; Bjerg et al., Reference Bjerg, Eggum, Jacobsen, Otte and Sorensen1989). Reduced CTTAD of DM was due to negative effect of TGLS on digestion (Duncan and Milne, Reference Duncan and Milne1990), whereas the increased CTTAD of protein on MM incorporation could be the influence of better amino acid balance of MM (De Blas et al., Reference De Blas, Faga, Rodriguez and Mendez1984). Interestingly, on 80 MM and 160 MM diets rabbits showed better nitrogen utilisation efficiency than on SBM diet. Possibly, these diets had a better combination of amino acid than that of either control (0 MM) that contained SBM or 245 MM that had MM as the sole protein source. It is hypothesised that glucosinolate may not have a deleterious effect on nitrogen utilisation.
Anti-nutritional factors such as resistant fibre, lignin and tannins supply have been implicated to influence intestinal characteristics and activity of the caecal ecosystem (Blas et al., Reference Blas, Cervera and Fernandez1994; De Blas et al.,Reference De Blas, Garcia and Carabaño1999; Gidenne, Reference Gidenne1997; Bennegadi et al., Reference Bennegadi, Gidenne and Licois2001). MM incorporation did not affect empty caecum weight, total caecum weight and intestine weight as per cent of LW, showing that the fibre quality of MM was as good as SBM. Linearly reduced caecum content weight with increasing MM-incorporated diets was probably due to better microbial activity in the caeco-colic segment of the rabbit digestive tract on MM-incorporated diets. MM has higher sulphur content (Papas et al., Reference Papas, Ingalls and Cansfield1978, Tyagi et al., Reference Tyagi, Tripathi and Karim1996) and sulphur is known to improve microbial activity in the intestine. Better microbial activity also supported by higher NH3-N and TCA-N content of caecal matter, and also by the improved CTTAD of DM and CP. The intestine and caecal fermentation characteristics of the present study are in agreement with the observations reported by Prasad et al. (Reference Prasad, Misra, Sankhyan, Mishra, Tripathi, Karim and Jakhmola2004), Gidenne et al. (Reference Gidenne, Jehl, Segura and Michalet-Doreau2002) and Carabaño et al. (Reference Carabaño, Motta-Ferreira, De Blas and Fraga1997).
The animals were in excellent condition throughout the experiment as evident by lack of any apparent sign of ill health. Feeding MM to rabbits did not affect their health and growth, although TGLS was reported to cause health and production problems. However, the adverse effect of dietary TGLS varies due to its level, feeding duration, animal species, age and sex (Tripathi and Mishra, Reference Tripathi and Mishra2007). Pigs fed a diet containing glucosinolate induced iodine deficiency and hypothyroid pigs had reduced bone and serum Zn content and serum alkaline phosphatase activity. Enlarged liver due to glucosinolate toxicity accompanied reduced RBC counts, haemoglobin (Hb) and haematocrit (Hc) in blood (Schone et al., Reference Schone, Winnefeld, Kirchner, Grun, Ludke and Hennig1990). Haematology and blood composition data were used as an indication of the health status of experimental animals. During the experiment, all the blood values recorded were within the normal range of reference for animals of similar age groups. However, the increased activity of AST and reduced WBC counts, and increased leucocyte counts showed that the MM incorporation impaired liver function and reduced immunity of rabbits fed MM diets, particularly those on the 245 MM diet. The TGLS degradation products are known to impair liver function and reduce the protein biosynthesis activities of liver (Barrett et al., Reference Barrett, Klopfenstein and Leipold1997; Tripathi et al., Reference Tripathi, Agrawal, Sharma and Mishra2001). The early cases of liver disease are clinically unapparent; however, they are detectable by elevation of liver enzymes in serum. Serum enzyme activities are generally elevated, an indicate hepatocyte damage. No significant differences were observed for the other hepatic enzyme activities (ALT, alkaline phosphatase), suggesting that the levels of TGLS in this study caused only a low and transient negative effect on hepatocyte. Feeding 245 MM diet to rabbits depressed their growth; in general, meat rabbits are marketed between 10 and 12 weeks of age so this is a short period of expression of deleterious effects of TGLS.
Conclusion
MM incorporated at 80, 160 and 245 g/kg in complete feed could replace SBM protein in growing-rabbit diets. MM inclusion up to 160 g/kg while replacing 66% of SMB protein in growing-rabbit diets had little effect on digestion, energy and protein utilisation, growth, caecal fermentation characteristics and blood composition. However, when SBM was wholly replaced by MM, negative effects on rabbit performance were observed. Although growing rabbit fed diets containing 160 g MM tolerated 8.4 mg TGLS per g diet during the active-growth phase, further studies are still required to confirm these inclusion levels and long-term feeding experiments shall provide valuable information on the glucosinolate tolerance of rabbits.