Introduction
The livestock sector has a significant contribution to the national economy of Ethiopia. However, production per animal is extremely low. The average lactation milk production for the indigenous cows ranges from 494 to 850 kg under optimum on-station management conditions (EARO, 1999).
To meet the ever-increasing demand for milk and milk products in Ethiopia, genetic improvement of the indigenous cattle has been proposed as one of the options. Genetic improvement of the indigenous cattle, basically focusing on crossbreeding as a quick way of increasing milk production, has been practiced for the last five decades. The use of crossbreds for milk production was based on earlier documented recommendations by Institute of Agricultural Research (IAR) (1982). A large cattle crossbreeding experiment was conducted across four environmentally diverse locations, namely Holetta, Bako, Adami Tulu and Melka Werer, in Ethiopia. The crossbreeding involved three indigenous breeds (Boran, Horro and Barka) and three exotic breeds (Holstein, Jersey and Simmental). The major recommendation of this effort was that the Holstein crosses were better than the others in milk production traits and that crosses of around 50% exotic inheritance could be used under favorable environmental and management conditions. On the other hand, by the virtue of being smaller in body size and more heat tolerant, the Jersey crosses have relative advantage over the Holsteins where nutrition is a limiting factor (IAR, 1982). Following this pioneer recommendation, a number of Government and non-Government organizations were involved in crossbreeding. Unfortunately, at a national level, no breeding policy was clearly defined as regards the level of exotic inheritance and the breed type to be used for the different climatic conditions and scenarios of the country. Data collected for a long time on crossbreeding studies by different institutions has not been systematically analyzed and documented to help in the design of sound and sustainable breeding program. Indeed, some studies compared indigenous cattle breeds with their contemporary crosses for dairy performance in Ethiopia (IAR, 1982; Kiwuwa et al., Reference Kiwuwa, Trail, Kurtu, Getachew, Anderson and Durkin1983; Haile-Mariam et al., Reference Haile-Mariam, Banjaw, Gebre-Meskel and Ketema1993; Negussie et al., Reference Negussie, Brannang, Banjaw and Rottmann1998; Demeke et al., Reference Demeke, Neser and Schoeman2004). Some workers (Haile-Mariam et al., Reference Haile-Mariam, Banjaw, Gebre-Meskel and Ketema1993; Demeke et al., Reference Demeke, Neser and Schoeman2004) also estimated genetic parameters for the economic traits.
Accurate estimation of breed additive and non-additive effects and separation into their causal components is essential for the design of a breeding program which fully exploits the value of crossbreeding (Cunningham and Syrstad, Reference Cunningham and Syrstad1987). In Ethiopia, however, limited studies (Demeke et al., Reference Demeke, Neser and Schoeman2004; Million and Tadelle, Reference Million and Tadelle2004) estimated these crossbreeding parameters. Documented information on crossbreeding is scarce to base sound and sustainable breeding programs. A need exists for more data to be compiled and analyzed to help in the design of breeding strategy. This study, therefore, was carried out with the following objectives: (i) to study the milk production performance of Ethiopian Boran and their crosses with Holstein in central Ethiopia; (ii) to estimate genetic parameters of milk production traits; (iii) to estimate crossbreeding parameters in Ethiopian Boran–Holstein crosses and (iv) to suggest breeding strategy for dairy improvement.
Material and methods
Source of data
Data for the study were collected from experimental dairy cattle herds of Ethiopian Boran and Ethiopian Boran–Holstein crossbred cattle maintained at the Debre Zeit Research Station of the International Livestock Research Institute (ILRI) and at the Holetta Agricultural Research Centre of the Ethiopian Institute of Agricultural Research (EIAR). Five genetic groups (Ethiopian Boran (0%), 50%, 62.5%, 75% and 87.5% of Holstein inheritance) represented in the two stations were used. Fifteen years (1990 to 2004) of data were used for this study.
Description of the farms
The Debre Zeit Research Station of the ILRI is located on the outskirts of the town of Debre Zeit, about 50 km south-east of Addis Ababa, in the Ethiopian highlands (9°N and 39°E), at an altitude of about 1850 m above sea level. Average annual rainfall in the Debre Zeit area is about 866 mm. The annual average temperature was 18.7°C and the average monthly relative humidity was 52.4%.
The Holetta Agricultural Research Centre is located 45 km west of Addis Ababa at 38.5°E longitude and 9.8°N latitude, and elevation of 2400 m above sea level. It is situated in the central highlands of Ethiopia. The average annual rainfall is about 1200 mm.
Animal management practices
The cattle in Debre Zeit farm were not grazed because of problem of tick infestation. Thus, they were all stall-fed. Clean water, hay and mineral lick were provided ad libitum. Additionally, animals had free access to teff (Eragrostis tef) straw. The animals were supplemented with concentrate mixture composed of wheat bran, noug seed cake (Guizoita abysinica) and molasses, based on milk production, two times per day. All calves were weighed at birth and allowed to suckle their dams for the first 24 h in order to obtain colostrum, after which they were moved to individual calf pens for bucket feeding (3 l milk per day) until weaning (57 days). Milking was done by hand twice a day (morning, 5:00 am and evening, 5:00 pm). Culling was based on production (low producers), age (old age) and health problems. Disease control was practiced through combined health management practices that included vaccination for the major diseases (black quarter, anthrax, contagious bovine pleuro pneumonia, pasteurellosis and foot and mouth disease), regular deworming (every 6 months) and treatment as diseases occurred.
The herd at Holetta was grazed on natural pasture for about 8 h during daytime. At night all animals were housed and supplemented with natural pasture hay conserved from part of the grazing area. Except for the lactating cows, which were supplemented with approximately 3–4 kg of concentrate at each milking, no other animal received any regular concentrate supplement. Occasionally, during the long-dry period and based on the condition of the animals, dry and young stocks were supplemented with an unspecified amount of concentrate. All animals had free access to clean water. Cows and heifers were all reared in a similar environment with fairly constant management. All calves were weighed at birth and allowed to suckle their dams for the first 24 h in order to obtain colostrum, after which they were moved to individual calf pens for bucket feeding until weaning at 90 days of age. Each calf was fed a fixed total of 260 kg of whole milk during the pre-weaning period. Weaned calves were kept indoors until the age of 6 months, during which they were fed ad libitum on natural pasture hay and supplemented with approximately 1 kg per day per animal of concentrate composed of 30% wheat bran, 32% wheat middling, 37% noug seed cake (G. abysinica) and 1% salt. At 6 months of age, all animals were grazed in a group on natural pastures for about 8 h a day and supplemented with conserved natural pasture hay at night.
The cows used in this study were the progeny of 448 dams and 72 sires. Of the total number of bulls used, 15 sires had progenies in both herds. All cows were sired by artificial insemination acquired from the National Artificial Insemination Center of Ethiopia.
Management of the two herds is not typical of what most smallholder farmers could achieve. The level of husbandry under smallholder cattle production system, unlike the situation in the two herds used for the present study, is characterized by the prevalence of many diseases, feed shortage and lack of skill on modern practices (Mohamed et al., Reference Mohamed, Simeon and Yemesrach2004). Therefore, results of the present study should be interpreted with an intensive dairy farm in mind.
Data editing and analysis
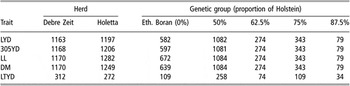
For purposes of this study, each lactation record was considered normal if a cow had produced milk for at least 60 days and terminated with registered voluntary drying-off date. Lactations truncated at day 60 were also excluded from the 305-day milk yield (305YD) analysis. The truncation point of 60 days was based on the recommendation of Kiwuwa et al. (Reference Kiwuwa, Trail, Kurtu, Getachew, Anderson and Durkin1983) for the indigenous Ethiopian cattle and their crosses. The acceptable lactation length (LL) for Zebu breeds is not well established and exclusions of short lactations were reported to minimize the genetic variance for milk yield (Madalena, Reference Madalena1988), although Mackinnon et al. (Reference Mackinnon, Thorpe and Baker1996) reported that inclusion or exclusion of short lactation had no significant effect on estimation of genetic variance and crossbreeding parameters. The animals that have abnormal calving, i.e., abortion and stillbirths, were not included in the analysis of breeding data. The data used for analysis are summarized in Table 1.
Number of records (from 584 cows) used for the analysis

LYD = lactation milk yield; 305YD = 305-day milk yield; LL = lactation length, DM = milk yield per day of lactation; LTYD = lifetime milk yield.
Traits studied were lactation milk yield (LYD), 305YD, LL, milk yield per day of lactation (DM) and lifetime milk yield (LTYD, the total milk produced by a cow from the initiation of first lactation till the day of last completed lactation).
The statistical analysis involved three steps. Firstly, least-squares analysis was carried out to compare the different genotypes and examine other fixed effects (SAS, 2002). The fixed effects fitted were as follows: genotype (five classes: Ethiopian Boran, 50%, 62.5%, 75% and 87.5% of Holstein inheritance); periods of calving (year group) (five classes: 1990–1992, 1993–1995, 1996–1998, 1999–2001 and 2002–2004); cow parity (five classes: 1, 2, 3, 4 and 5+), calving season, grouped into three classes, based on the pattern of annual rainfall distribution in the area (November to February: dry period; March to June: light rains and July to October: main rainy season) and herd (two classes: Debre Zeit and Holetta). Sire effect, unfortunately, was not fitted as random effect because not many sires had daughters over the two herds. Thus, a fixed effect model was fitted. In preliminary analysis, year effect was fitted individually. However, no consistent and meaningful variation was observed over the years. As a result year was grouped into period consistent with trends in management of the herds. The two-way interactions of effects were also fitted in the models and retained in the final model when found significant (P < 0.05) in the preliminary analysis. However, results of the interaction effects are not presented. The Tukey–Kramer test was used to separate least-squares means with more than two levels.
Secondly, (co)variance components and the resulting genetic and phenotypic parameters (heritability, genetic correlations and repeatability) were estimated using the derivative-free restricted maximum likelihood (DFREML) computer package of Meyer (Reference Meyer1998). A repeatability animal model was fitted, where direct additive effects plus permanent environmental effect due to repeated records per cow were fitted as random effects except for LTYD where direct additive effect was the only random effect fitted. The fixed effects fitted in the least-squares analysis were fitted for crosses but genotype had four classes (50%, 62.5%, 75% and 87.5% of Holstein inheritance). Sires of all crosses were Holstein. For Ethiopian Boran all fixed effects except genotype were fitted. The convergence criterion for the variance component estimates was 10−7. A maximum of 900 iterations were carried out for the convergence.
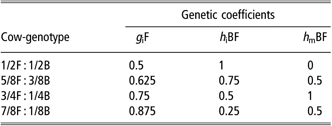
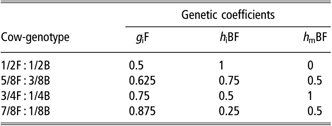
Thirdly, multiple regression analysis (SAS, 2002) was used to estimate crossbreeding parameters. For the regression analysis, coefficients of expected breed content and heterozygosity in the cow (Table 2) were fitted as covariates to obtain estimates of the individual additive (g iF), individual heterosis (h iBF) and maternal heterosis (h mBF) effects using similar procedures to those of Hirooka and Bhuttyan (Reference Hirooka and Bhuttyan1995) and Kahi et al. (Reference Kahi, Mackinnon, Thorpe, Baker and Njubi1995). Expected heterozygosity with respect to the genes of two breeds was calculated as the expected proportion of genes from the sire and dam, which differed with respect to the two breeds. For example, the expected heterozygosity with respect to genes of the Ethiopian Boran (B) and Holstein (F), h iBF, was calculated as (g sB*g dF) + (g sF*g dB), where the superscripts s and d denote that the genes come from the sire and the dam, respectively. Similarly, expected heterozygosity with respect to two breeds was calculated for the genotype of the dam of cow and was denoted as h mBF. Breed additive effects of, for example, F were calculated using the formula g iF = ½(g sF + g dF). The breed additive effects for Holstein were estimated as deviations from the Ethiopian Boran breed. Thus, the full model included effects of g iF, h iBF and h mBF as well as fixed effects described in the least-squares analysis except for the genetic group.
Genetic coefficients for breed additive (g iF), individual heterosis (h iBF) and maternal heterosis (h mBF) in crossbreds
Results
Fixed effects and genotype comparisons
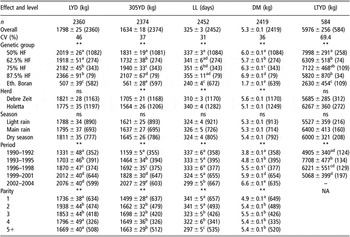
Least-squares means and standard errors for fixed effects are summarized in Table 3. The genetic groups significantly (at least P < 0.05) differed in all the milk production traits considered (LYD, 305YD, LL, DM and LTYD). Ethiopian Boran cattle were consistently inferior (P < 0.01) to all the Ethiopian Boran–Holstein crosses in all the dairy traits studied. When the crosses with different levels of exotic inheritance were compared, LYD, 305YD and DM were significantly (P < 0.01) higher for 75% and 87.5% crosses compared to 50% and 62.5% ones. It was observed that as the exotic inheritance level increased, all the traits showed an increasing trend. However, when the LTYD was studied it was the 50% crosses that had significantly (P < 0.01) higher values than all the other genetic groups.
Least-squares means (±s.e.) for effects of genetic group, herd, period, season and parity on milk production traits

LYD = lactation milk yield; 305YD = 305-day milk yield; LL = lactation length, DM = milk yield per day of lactation; LTYD = lifetime milk yield; CV = coefficient of variation; HF = Holstein Friesian.
*P < 0.05; **P < 0.01; ns = non-significant; NA = not applicable.
Least-squares mean with same superscript in the same column indicate non-significance.
Numbers in parenthesis indicate number of records.
Herd effect was not significant (P > 0.05) for LYD and LTYD. However, herd was found to have effect (P < 0.01) on 305YD, LL and DM. The 305YD and DM were higher for the Debre Zeit herd than for the Holetta herd. But, LL was higher for the Holetta herd. Season of calving did not have effect (P > 0.05) on all milk production traits.
Milk production traits showed an increasing trend over the periods, while LL declined. The increase in milk production traits over periods was quite substantial. For example, an increase of 745 kg of LYD from the first period (1990–1992) to the fifth period (2002–2004) was recorded. The same has occurred for 305YD, DM and LTYD. On the other hand, LL dropped from 337 days in the first period to 299 days in the fifth period. As expected, parity had a significant (P < 0.01) effect on milk production traits. Cows that calved for the first time had significantly lower LYD, 305YD and DM, but longer LL, than all the other parities.
Estimates of genetic parameters
Heritability
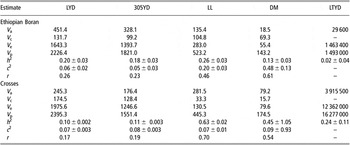
Variance components and estimates of heritability for milk production traits are summarized in Table 4. Heritability estimates of LL for Ethiopian Boran and crosses were 0.26 ± 0.03 and 0.63 ± 0.02, respectively. Heritability of 305YD for Ethiopian Boran and crosses was estimated at 0.18 ± 0.03 and 0.11 ± 0.003, respectively. The corresponding values for LYD were 0.20 ± 0.03 and 0.10 ± 0.002, respectively. The estimates for DM for the two genetic groups were rather high. Heritability for LTYD was estimated at 0.02 ± 0.04 and 0.24 ± 0.11 for Ethiopian Boran and crosses, respectively.
Estimates of variance components, heritabilities (h 2 ± s.e.), repeatability (r) and cow effects (c 2 ± s.e.) for milk production traits

LYD = lactation milk yield; 305YD = 305-day milk yield; LL = lactation length, DM = milk yield per day of lactation; LTYD = lifetime milk yield; V a = additive genetic variance; V c = permanent environmental variance; V e = residual variance; V p = phenotypic variance.
Repeatability
Repeatability estimates in Ethiopian Boran and crosses (Table 4) for LL (0.46 and 0.70, respectively) and DM (0.61 and 0.54, respectively) were high. The corresponding estimates for 305YD (0.23 and 0.19, respectively) and LYD (0.26 and 0.17, respectively) were, however, very low.
Genetic correlations
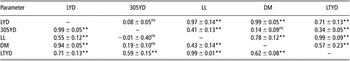
Genetic correlations between milk production traits for Ethiopian Boran and crosses are summarized in Table 5. In crossbred cattle, LL had significant (at least P < 0.05) genetic correlation with all milk production traits, the strongest genetic correlation of a near-unity (0.99 ± 0.01) being estimated with LTYD. The genetic correlations of LL with other milk production traits in Ethiopian Boran were more or less similar to those of crosses, except for a non-significant (P > 0.05) genetic correlation between LL and 305YD (−0.01 ± 0.40). LYD had strong and significant (at least P < 0.05) genetic correlation with 305YD, DM and LTYD in both genetic groups. 305YD had low and non-significant (P > 0.05) genetic correlation with DM in both the genetic groups.
Genetic correlations (and s.e.) between milk production traits for Ethiopian Boran (above diagonal) and their crosses (below diagonal)

LYD = lactation milk yield; 305YD = 305-day milk yield; LL = lactation length, DM = milk yield per day of lactation; LTYD = lifetime milk yield.
*P < 0.05; **P < 0.01; ns = non-significant.
Crossbreeding parameters
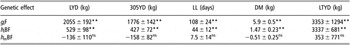
The individual additive genetic breed difference for milk production traits was all significant (P < 0.01). The estimates, in favor of Holstein, were 2055 kg for LYD, 1776 kg for 305YD, 108 days for LL, 5.9 kg for DM and 3353 kg for LTYD (Table 6). Crossbreeding of the Holstein with the Ethiopian Boran resulted in desirable and significant (P < 0.01) individual heterosis for all milk production traits (Table 6). These estimates, obtained as a deviation of F1 mean values from the mid-parent mean values, are 529 ± 98, 427 ± 72 kg, 44 ± 12 days, 1.47 ± 0.23 and 3337 ± 681 kg, for LYD, 305YD, LL, DM and LTYD, respectively. The maternal heterotic effects were non-significant (P > 0.05) for all traits.
Estimates of breed additive (g iF), individual heterosis (h iBF) and maternal heterosis (h mBF) for milk production traits

LYD = lactation milk yield; 305YD = 305-day milk yield; LL = lactation length, DM = milk yield per day of lactation; LTYD = lifetime milk yield.
*P < 0.05; **P < 0.01; ns = non-significant.
Discussion
Crossbreeding indigenous Ethiopian Boran with Holstein had resulted in improvement of milk production performance traits. For example, 50% Holstein crosses had a four-fold increase over the Ethiopian Boran breed in terms of LYD, 305YD, DM and LTYD; they were also milked for 97 more days than Ethiopian Boran. Except for the magnitude of differences, the superior performance of crossbred progeny compared with the Ethiopian Boran for milk production traits is as expected and is in agreement with comparative results reported for Bos indicus and their crosses with European dairy breeds in the tropics (IAR, 1982; Kiwuwa et al., Reference Kiwuwa, Trail, Kurtu, Getachew, Anderson and Durkin1983; Thorpe et al., Reference Thorpe, Kangethe, Rege, Mosi, Mwandotto and Njuguna1993; Rege et al., Reference Rege, Aboagye, Akah and Ahunu1994; Udo et al., Reference Udo, Mgeni and Syrstad1995; Demeke et al., Reference Demeke, Neser and Schoeman2004).
When the crosses were compared, it was observed that as the exotic inheritance level increased, LYD, 305YD and DM showed an increasing trend. However, LTYD was higher in 50% crosses than in all the other genetic groups. This was associated with longer productive herd life of the 50% crosses compared with others (data not shown). The results of this analysis concur with those of other studies in the tropics (Rege, Reference Rege1998; Million and Tadelle, Reference Million and Tadelle2003). Rege (Reference Rege1998) summarized results from 80 reports in the literature on crossbreeding in the tropics to study the relationship between dairy performance and proportion of exotic genes, and found that grades higher than 1/2 exotic did not perform any worse than the F1, in all traits, except for calving interval, which was longer in higher grades. The results showed consistent increase in milk yield with increasing levels of exotic genes up to 50% exotic inheritance. Indeed, 7/8 and pure exotic genotypes tended to be superior in milk yield. Additionally, studies in Brazil (Madalena, Reference Madalena1981) have shown that the F1 generally had higher milk yield and shorter calving interval, but that their superiority over higher grades declined as the production level increased in response to improved production environment. The superiority in the present study of higher levels of exotic inheritance could, therefore, be attributed to the rather better management practiced in these herds. However, these results should be interpreted cautiously because when the overall benefit, as measured by lifetime milk production, is considered, the 50% crosses were superior. Similar results have also been observed in a number of other studies in Africa (Negussie et al., Reference Negussie, Brännäng and Rottmann1999) and elsewhere (Vaccaro, Reference Vaccaro1990; Sahota and Gill, Reference Sahota and Gill1991).
It is expected that being on different locations and having had different management practices, the two herds could vary in the level of performance for the milk production traits. However, the lack of consistent variation between the two herds would make it difficult to reach any definite conclusions. Indeed, influence of herd on milk production traits has been extensively documented even when standard and similar management practices were followed at all the farms (Jadhav et al., Reference Jadhav, Tripathi, Taneja and Kale1991; Mukherjee, Reference Mukherjee2005).
Season of calving had no significant effect on milk production performance traits. This does not agree with several studies (Raheja, Reference Raheja1994; Mukherjee, Reference Mukherjee2005), which indicated a significant influence of season of calving on milk yield traits. However, studies by Hirooka and Bhuttyan (Reference Hirooka and Bhuttyan1995) and Million and Tadelle (Reference Million and Tadelle2003) revealed that season of calving had not influenced (P > 0.05) many milk production traits of crosses of local and Holstein cows. Thus, it could be suggested that in the tropics, the influence of climatic conditions may be negligible under optimal feeding and management conditions.
Milk production traits showed an increasing trend over the periods, while LL declined. The increase in milk production performance over years may not only be caused by inter-annual random change of the climatic factors but also include management changes. Given the non-significant effect of calving season on milk production performance in the present study, it could be inferred that an improved management in the herds might have caused improvement in the performance traits. This result agrees well with other studies (Million and Tadelle, Reference Million and Tadelle2003; Demeke et al., Reference Demeke, Neser and Schoeman2004).
Cows that calved for the first time had lower LYD, 305YD and DM, but longer LL than all the other parities. The increase in LYD to the second parity and subsequent fall later obtained in the present study were similar to the pattern observed in both Ayrshire and Sahiwal herds in the Kenyan environment (Trail and Gregory, Reference Trail and Gregory1982), in Holstein cattle in Kenya (Rege, Reference Rege1991) and in Frieswal cattle in India (Mukherjee, Reference Mukherjee2005). But in the present study, LYD peaked numerically at the second lactation unlike the other studies where the peak was at later parities. For 305YD and DM, no difference (P > 0.05) was recorded between the second and subsequent parities. Significant changes in milk production for parity effect were also reported by Thorpe et al. (Reference Thorpe, Kangethe, Rege, Mosi, Mwandotto and Njuguna1993), Rege et al. (Reference Rege, Aboagye, Akah and Ahunu1994) and Demeke et al. (Reference Demeke, Neser and Schoeman2004).
In general, the moderate heritability estimates for milk production traits (except for LTYD in Ethiopian Boran) indicate that sufficient additive genetic variance exists for these traits that could be used for selection within each genetic group/breed population in conjunction with crossbreeding. Comparison between the genetic groups (Ethiopian Boran v. crosses) for heritability estimates of milk production traits did not follow a strict trend. For LYD and 305YD, heritability estimates were larger in Ethiopian Boran. For the other three traits the values were higher in crosses. Because of a relatively weak selection and thus broadened genetic base in Ethiopian Boran than in crosses, large additive genetic variance is expected in the former. However, the heritability estimates recorded do not support this proposition.
Repeatability estimates in Ethiopian Boran and crosses for LL and DM were high and indicated that culling of animals on the basis of performance in early lactations could be carried out with a reasonable degree of accuracy. The corresponding estimates for 305YD and LYD were, however, very low. Thus, temporary environmental factors contributed appreciably to the variation in 305YD and LYD among parities; hence, cows should not be culled on single (or only few) initially available records of 305YD and LYD.
With the exception of associations between 305YD and DM, the correlation estimates between various milk production traits are strong and within the range of reported estimates in the literature (Lobo et al., Reference Lobo, Madalena and Vieira2000; Demeke et al., Reference Demeke, Neser and Schoeman2004; Mukherjee, Reference Mukherjee2005). Therefore, genetic improvement targeted at one of the traits should result in a desirable correlated response to selection in the other trait.
The breed additive contributions of the Holstein breed for milk production traits are generally higher than the corresponding estimates reported for this breed elsewhere in the tropics (Sharma and Pirchner, Reference Sharma and Pirchner1991; Thorpe et al., Reference Thorpe, Kangethe, Rege, Mosi, Mwandotto and Njuguna1993). For example, Sharma and Pirchner (Reference Sharma and Pirchner1991), utilizing data obtained from a number of dairy farms in India, have reported a 773 kg difference in LYD between Holstein and Sahiwal. Thorpe et al. (Reference Thorpe, Kangethe, Rege, Mosi, Mwandotto and Njuguna1993) also reported that the additive contribution to LYD of Sahiwal was 746 kg less than that of Bos taurus (Ayrshire and Friesian). The differences in these estimates might be a result of the lower milk production of the Ethiopian Boran breed compared with other milking-type tropical indigenous cattle, such as the Sahiwal, which was commonly used in several other crossbreeding studies (Cunningham and Syrstad, Reference Cunningham and Syrstad1987; Mackinnon et al., Reference Mackinnon, Thorpe and Baker1996). Demeke et al. (Reference Demeke, Neser and Schoeman2004), on the other hand, reported a comparable additive breed effect in the crosses of Holstein and Ethiopian Boran in Ethiopia. The estimates for individual heterosis effects are within the range of reported heterotic effects for milk production traits of other B. taurus × B. indicus crosses (Sharma and Pirchner Reference Sharma and Pirchner1991; Thorpe et al., Reference Thorpe, Kangethe, Rege, Mosi, Mwandotto and Njuguna1993; Rege et al., Reference Rege, Aboagye, Akah and Ahunu1994; Mackinnon et al., Reference Mackinnon, Thorpe and Baker1996; Rege, Reference Rege1998, Demeke et al., Reference Demeke, Neser and Schoeman2004).
Conclusion
Milk production performance of Ethiopian Boran was found to be consistently inferior to the crosses. Commercial milk production has been improved by crossing Ethiopian Boran and Holstein breeds because of the additive genetic contribution of the Holstein and its heterotic effects. Favorable genetic association existed between milk production traits (except for some traits), and the heritability of the traits was also generally moderate to high (except for LTYD in Ethiopian Boran). Therefore, selection within each of the genetic groups and crossbreeding should substantially improve the milk production potential of the indigenous Ethiopian Boran breed under such production systems. Higher exotic inheritance levels (for example, 87.5% Holstein) could be justified under such intensive production systems. As the level of management achievable under most smallholders condition in Ethiopia is rather unfavorable to higher exotic inheritance levels, the recommendation made earlier (IAR, 1982), that is around 50% Holstein inheritance, should be adhered to. Indeed, maintaining 50% Holstein inheritance under field conditions is difficult. Strategies (for example, the one suggested by Philipsson et al., Reference Philipsson, Rege and Okeyo2006) should be designed to result in 50% composition of each of the two breeds.
Acknowledgments
We sincerely thank ILRI and EIAR for provision of data. The senior author wishes to thank the Jimma University for granting him study leave and ILRI for research facilities.