



Introduction
For most insects, diapause is a common survival strategy to adapt to adverse environmental conditions such as extreme temperatures, food scarcity, and drought (Gill et al. Reference Gill, Goyal and Chahil2017). The use, accumulation, and conversion of nutrients affect insect diapause (Ren et al. Reference Ren, Qi, An, Han and Chen2016). During diapause, a series of physiological and biochemical changes occur in insects, including the specific accumulation or conversion of endogenous nutrients such as lipids, proteins, and carbohydrates, to guarantee the survival of diapause individuals in adverse environments and their energy needs for post-diapause development (Hahn and Denlinger Reference Hahn and Denlinger2007, Reference Hahn and Denlinger2011). Diapause individuals often experience a decline in moisture content, a rise in fat content, and the cessation of RNA and DNA synthesis, and some insects also exhibit a rise in amino acid and protein contents (Danks Reference Danks1987). As such, investigating changes in the content of biochemical substances related to diapause in insects can improve our understanding of the mechanisms underlying insect diapause.
Diapause individuals generally need little or no feeding and survive through long diapause periods by regulating the distribution of nutrients in vivo. Insects, such as Rhagoletis pomonella (Diptera: Tephritidae) (Ragland et al. Reference Ragland, Egan, Feder, Berlocher and Hahn2011), inhibit metabolism and respiration during diapause to reduce nutrient consumption. Moreover, by regulating nutrient conversion, insects enhance their stress resistance and sustain their survival during diapause. For example, Culex pipiens (Diptera: Culicidae) undergoes significant carbohydrate–lipid conversion during diapause to satisfy the energy needs of individuals (Zhou and Miesfeld Reference Zhou and Miesfeld2009). Leptinotarsa decemlineata (Coleoptera: Chrysomelidae) needs no feeding during diapause but feeds heavily before diapause, exhibiting characteristics such as high metabolic rate and expression of specific genes (Yocum et al. Reference Yocum, Buckner and Fatland2011). In the case of Carposina sasakii (Lepidoptera: Carposinidae), significant changes occur in biochemical parameters such as fats, glucose, and mannitol during the post-diapause development period (Zhang et al. Reference Zhang, Peng, Zhao, Hoffmann, Li and Ma2016).
Coridius chinensis (Dallas) (Hemiptera: Dinidoridae) is known for its dual use as medicine and food (Hou Reference Hou2019; Bonysana et al. Reference Bonysana, Singh, Devi, Koijam, Kapesa and Kalita2024). It has been reported that Coridius chinensis has pharmacological actions in rodents and in cells in vitro, such as antioxidant activity, anti-inflammatory effects, reproductive protection, antibacterial activity, anticancer properties, and promotion of angiogenesis effects (Li et al. Reference Li, Zhao and Du2015; Liu et al. Reference Liu, Cen, Fu, Wang, Wang, Xu and Hou2019; Cen et al. Reference Cen, Wang, Xiong, Jiang and Hou2022; Bonysana et al. Reference Bonysana, Singh, Devi, Koijam, Kapesa and Kalita2024; Cai et al. Reference Cai, Chen, Khan, Li, Tan and Tian2024; Luo et al. Reference Luo, Xiong, Wang, Cen, Liu and Wang2024), which make C. chinensis an important traditional medicine for treating various conditions and diseases, including impotence, infertility, gastric cancer, liver cancer, and hemangioma in China and India (Liu Reference Liu2002; Hou et al. Reference Hou, Sun and Li2012; Bonysana et al. Reference Bonysana, Singh, Devi, Koijam, Kapesa and Kalita2024; Xiong et al. Reference Xiong, Zeng, Lei, Wei, Zhou and Hou2024). The distribution of C. chinensis is mainly limited to Sichuan, Guizhou, and Yunnan provinces in China, with a reproduction rate of only one generation per year. Post-eclosion adults start overwintering diapause and stop food intake in October, lasting until early May of the following year when they migrate from overwintering sites to crops such as chayotes (Cucurbitaceae) and pumpkins (Cucurbitaceae) for feeding and breeding. Thus, the long diapause period, of up to eight months (Wei et al. Reference Wei, Shu, Luo and Gou2015; Ji et al. Reference Ji, Chen, Li, Lou, Liu, Dai and Shi2022), seriously restricts the culture and use of C. chinensis for traditional medicine. To clarify dynamic changes in the physiological characteristics of C. chinensis between the diapause and post-diapause development periods and to explore how physiological and biochemical changes are related to diapause, this study investigated changes in the moisture, fat, carbohydrate, and protein content of C. chinensis between the diapause and post-diapause development periods, providing a scientific basis for further research on the diapause physiology of C. chinensis.
Materials and methods
Test insect
Adult C. chinensis in the overwintering diapause stage were collected from an overwintering site near a vegetable field in the Housuo Community of Hongta District (24° 26′ N, 102° 32′ E; altitude: 1667 m), Yuxi, China, from October 2021 to April 2022. During this period, test insects were gathered from the designated site in the middle of each month. The post-diapause adult C. chinensis were captured from the chayotes grown in a vegetable field in the same community in mid-May 2022. Male and female insects can be distinguished by the end of abdomen and the special structure on the tibiae of hind leg in females.
Chemicals
Anthrone, trichloroacetic acid, and Coomassie brilliant blue G250 were purchased from Shanghai Macklin Biochemical Co. Ltd. (Shanghai, China). Anhydrous ethanol, glucose, sodium sulfate, sulfuric acid, sodium hydroxide, and sodium chloride were purchased from Aladdin Scientific (Shanghai).
Determination of moisture content
The moisture content of each of at least male and female C. chinensis adults was determined gravimetrically. A total of 40 flat weighing bottles from Changde Bkmam Biotechnology Co. Ltd. (Changde, China) was washed clean, marked at the mouth of bottles with a marker, and oven-dried at 65 °C for three hours. After that, the bottles were transferred to a dryer, allowed to cool to room temperature (about 1 hour), and then weighed (M0). One adult C. chinensis was placed into each weighed bottle, which was weighed again (M1). The weighing bottles containing C. chinensis were dried at 65 °C for nine hours, allowed to cool to room temperature in a dryer, and weighed (M2). The bottles were dried repeatedly until a constant weight was achieved. The moisture content (W) of each C. chinensis was calculated using the following formula:
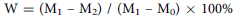
Determination of fat content
The fat content of each of at least three male and female C. chinensis adults was determined by the Soxhlet extraction method. The weighed dry insect (m) was ground well, placed in a fat-free filter paper bag, dried at 105 °C for two hours to a constant weight, numbered, and weighed again (m1). Before extraction, the sample to be tested was soaked in anhydrous ethanol in an extraction tube for 12 hours, followed by extraction at around 17 5 °C for nine hours. After extraction, the filter paper bag was collected and oven-dried at 105 °C to a constant weight, cooled in a closed container, and weighed (m2). The fat content (Fa) of C. chinensis was calculated using the following formula:
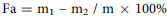
Determination of glycogen and trehalose content
The glycogen and trehalose content levels of each of at least three male and female C. chinensis adults were determined via anthrone colorimetry, according to the method by Yi (Reference Yi2007) but with slight modifications.
Standard curve generation
Six test tubes were set for 0, 0.2, 0.4, 0.6, 0.8, and 1.0 mL of a standard glucose solution (0.1 mg/mL), and the solutions were topped up to 2 mL with distilled water, followed by the addition of 8 mL of a temporarily prepared anthrone reagent. The test tubes were then cooled in an ice-water bath for 10 minutes and heated in a boiling-water bath for 20 minutes. After that, the test tubes were cooled with tap water and allowed to stand at room temperature for 10 minutes. The optical-density value at 620 nm was measured three times using a dual-beam UV-visible spectrophotometer (model: TU-1901, Beijing Puxi General Instrument Co., Ltd., Beijing, China). The standard curve was generated using the concentration of the standard glucose solution (mg/mL).
Determination of glycogen content
A single dry insect was put into a mortar, and 10 mL of 10% trichloroacetic acid solution and a little quartz sand were added, and the contents were ground finely. The ground extract was transferred to a centrifuge tube, incubated at 4 °C for four hours, and centrifuged at 5000 revolutions/minute for five minutes. After the supernatant was collected, 10 mL of 10% trichloroacetic acid were added for a repeated extraction. After mixing the supernatants, 10 mL of the solution were mixed with 30 mL of 95% ethyl alcohol, and four drops of a saturated sodium sulfate solution were added. The mixture was then stored at 4 °C. After 3 days, the mixture was centrifuged at 3000 revolutions/minute for 20 minutes, and the supernatant was discarded. The precipitate was dissolved in 100 mL of redistilled water for later use. Subsequently, 2 mL of the test solution were placed in a test tube, which was then immersed in an ice-water bath, followed by the addition of 8 mL of the anthrone reagent and boiling in a boiling-water bath for 20 minutes. After cooling, the optical-density value at 620 nm was measured using a dual-beam UV-visible spectrophotometer.
Determination of trehalose content
A single dry insect was put into a mortar, and 5 mL of a 10% trichloroacetic acid solution and a little quartz sand were added, and the contents were ground finely. The ground extract was transferred to a centrifuge tube and centrifuged at 5000 revolutions/minute for five minutes. The supernatant was transferred to a 100-mL volumetric flask, and 10 mL of 10% trichloroacetic acid were added for a repeated extraction. The mixture then was centrifuged 5000 revolutions/minute for five minutes. The supernatants were mixed and diluted for later use to a volume of 100 mL using distilled water. Thereafter, 2 mL of the test solution were mixed with 4 mL of a 0.15% sulfuric acid aqueous solution, and the mixture was heated in boiling water for 10 minutes and cooled, followed by the addition of 4 mL of 30% sodium hydroxide solution and heating in boiling water for 10 minutes. After cooling, 2 mL of the mixture were mixed with 10 mL of the anthrone reagent, and the mixture was heated in boiling water for 20 minutes. After cooling, the optical-density value at 620 nm was measured using a dual-beam UV-visible spectrophotometer.
Determination of protein content
The protein content of each of at least four male and female C. chinensis adults was determined using the Coomassie brilliant blue method. The protein test solution was prepared according to the method by Yi (Reference Yi2007), with slight modifications.
Standard curve generation
Seven test tubes were set for 0.0, 0.2, 0.4, 0.6, 0.8, 1.2, and 1.6 mL of the prepared standard protein test solution, and the solutions were topped up to 2 mL with a 0.9% sodium chloride solution, followed by the addition of 8 mL of a temporarily prepared Coomassie brilliant blue G250 reagent (0.01%). After even mixing, the mixture was allowed to equilibrate at room temperature for three minutes. The first test tube (0.0 mL) was used as the blank control, and the optical-density value at 595 nm was measured using a dual-beam UV-visible spectrophotometer. The standard curve was drawn using the concentration of the standard protein solution (μg/mL) as the x-axis and the optical-density value as the y-axis.
Preparation and determination of the test solution
A single dry insect was put into a mortar, and 10 mL of a 0.9% sodium chloride solution and a little quartz sand were added, and the contents were ground finely. The ground extract was transferred to a centrifuge tube and centrifuged at 5000 r/min for 10 minutes. Centrifugation was repeated twice. The centrifuged supernatant was transferred to a volumetric flask and topped up to 100 mL with a 0.9% sodium chloride solution for later use. Thereafter, 2.0 mL of the test solution were evenly mixed with 8.0 mL of the Coomassie Brilliant Blue reagent, and the mixture was allowed to equilibrate at room temperature for three minutes. The optical-density value at 595 nm was measured using a dual-beam UV-visible spectrophotometer.
Data analysis
All data were presented as means ± standard error of the mean. One-way analysis of variance and then the least significant difference test were performed to analyse the differences in dynamic changes of moisture, fat, carbohydrate, and protein content levels using SPSS 25.0 software (IBM, Armonk, New York, United States of America). The differences in moisture, fat, carbohydrate, and protein contents between female and male were tested by the independent sample t-test (significance level: α = 0.05).
Results
Changes in the moisture content of C. chinensis between the diapause and post-diapause development periods
Significant differences in the moisture content of the adult C. chinensis occurred between the diapause and post-diapause development periods (F 7,312 = 39.474; P < 0.001; Fig. 1A). The moisture content of C. chinensis during diapause (from October 2021 to April 2022) presented a trend of initial increase, followed by a decrease over time. The moisture content at the beginning of diapause (October 2021, 466.65 ± 5.69 mg/g) was significantly lower than that at any other stage (P < 0.05), and the moisture content during post-diapause development period (May 2022, 616.37 ± 6.47 mg/g) was the highest, significantly higher than both that from October to December 2021 and that in February and April 2022 (P < 0.05). However, moisture content in male and female adults did not differ significantly in any stage (P > 0.05; Fig. 1B).
Dynamic changes in the moisture content of C. chinensis during the diapause and post-diapause periods: A, dynamic changes in moisture content of female and male; B, moisture content comparison between the male and female adult. Bars represent means ± standard error values. Different letters among the columns indicate significant differences (analysis of variance, P < 0.05). The number in the column represents the sample size. ns, not significant.

Changes in the fat content of C. chinensis between the diapause and post-diapause development periods
Significant differences in the fat content of the adult C. chinensis occurred between the diapause and post-diapause development periods (F 7,72 = 20.945; P = 0.041; Fig. 2A). The fat content of C. chinensis gradually declined over time. It was highest at the beginning of diapause (October 2021, 407.74 ± 11.38 mg/g), when it was significantly higher than that at any other stage except that of January 2022 (P < 0.05). The fat content during the post-diapause development period (May 2022, 103.98 ± 19.20 mg/g) was the lowest, when it was significantly lower than that during diapause (from October 2021 to April 2022; P < 0.05). Fat content in male and female adults did not differ significantly in any stage (P > 0.05; Fig. 2B).
Dynamic changes in the fat content of C. chinensis during the diapause and post-diapause: A, dynamic changes in fat content of female and male; B, fat content comparison between the male and female adult. Bars represent means ± standard error values. Different letters among the columns indicate significant differences (analysis of variance, P < 0.05). The number in the column represents the sample size. ns, not significant.

Changes in the glycogen content of C. chinensis between the diapause and post-diapause development periods
Significant differences in the glycogen content of the adult C. chinensis occurred between the diapause and post-diapause development periods (F 7,72 = 7.628; P < 0.001; Fig. 3A). The glycogen content of C. chinensis was lower during diapause (from October 2021 to April 2022) but rose sharply during the post-diapause development period (May 2022, 26.57 ± 8.70 mg/g), reaching a level significantly higher than that during diapause (P < 0.05). Glycogen content in male and female adults did not differ significantly at any stage (P > 0.05; Fig. 3B).
Dynamic changes in the glycogen content of C. chinensis during the diapause and post-diapause periods: A, dynamic changes in glycogen content of female and male; B, glycogen content comparison between the male and female adult. Bars represent means ± standard error values. Different letters among the columns indicate significant differences (analysis of variance, P < 0.05). The number in the column represents the sample size. ns, not significant.

Changes in trehalose content of C. chinensis between the diapause and post-diapause development periods
Significant differences in the trehalose content of the adult C. chinensis occurred between the diapause and post-diapause development periods (F 7,72 = 4.618; P < 0.001; Fig. 4A). The trehalose content of C. chinensis gradually declined in the early stages of diapause (from October to December 2021) and was followed by a significant increase in the middle stage (January 2022), a gradual decline in the late stage (from February to April 2022), and a significant increase during the post-diapause development period (May 2022). The trehalose content at the beginning of diapause (October, 17.06 ± 2.55 mg/g) was the highest – significantly higher than that from November to December 2021 and from March to April 2022 (P < 0.05). Trehalose content in male and female adults differed significantly only in January and April 2022 (P < 0.05), with the trehalose content of male adults being higher in each case (Fig. 4B).
Dynamic changes in the trehalose content of C. chinensis during the diapause and post-diapause periods: A, dynamic changes in trehalose content of female and male; B, trehalose content comparison between the male and female adult. Bars represent means ± standard error values. Different letters among the columns indicate significant differences (analysis of variance, P < 0.05). The number in the column represents the sample size. ns, not significant. *P < 0.05, **P < 0.01.

Changes in the protein content of C. chinensis between the diapause and post-diapause development periods
Significant differences in the protein content of the adult C. chinensis occurred between the diapause and post-diapause development periods (F 7,72 = 88.778; P < 0.001; Fig. 5A). The protein content of C. chinensis was low in the early stage of diapause (from October to December 2021) – significantly lower than that in the middle and late stages of diapause (from January to April 2022) and during the post-diapause development period (May 2022; P < 0.05). Protein content rose sharply in January 2022 and remained relatively higher until May 2022. The protein content at the beginning of diapause (October 2021, 6.53 ± 0.94 mg/g) was the lowest, and protein content levels in January (65.72 ± 3.56 mg/g) and March 2022 (70.84 ± 2.04 mg/g) were significantly higher than those in any other month (P < 0.05). Protein content in male and female adults differed significantly only in January and May 2022 (P < 0.05), with the protein content of male adults being higher in each case (Fig. 5B).
Dynamic changes in the protein content of C. chinensis during the diapause and post-diapause periods: A, dynamic changes in protein content of female and male; B, protein content comparison between the male and female adult. Bars represent means ± standard error values. Different letters among the columns indicate significant differences (analysis of variance, P < 0.05). The number in the column represents the sample size. ns, not significant. *P < 0.05.

Discussion
Insect diapause is a slow developmental process that is accompanied by the accumulation or conversion of related substances in vivo (Kostál Reference Kostál2006). During overwintering, diapause insects synthesise and accumulate various energy-storing and cold-resistant substances in their bodies, such as fats, carbohydrates, and proteins, to enhance their cold resistance and survive adverse environments (Hahn and Denlinger Reference Hahn and Denlinger2007). The results of the present study indicate significant differences in changes in the moisture, fat, carbohydrate, and protein contents of C. chinensis between the diapause and post-diapause development periods, with obvious stage characteristics, and that the differences between males and females were largely insignificant.
The moisture content of C. chinensis during diapause (from October 2021 to April 2022) presented an “inverted-V-shaped” trend over time. The moisture content at the beginning of diapause (October 2021) was significantly lower than that at any other stage, and the moisture content during the post-diapause development period (May 2022) was the highest (Fig. 1A) of both periods. In Yuxi area of Yunnan Province, C. chinensis migrates to the overwintering site in October every year; before leaving the host plant, the insect needs to accumulate a large amount of fat for the winter, as evidenced by the large number of fat granules we found in the abdominal cavity of each C. chinensis (unpublished data). Because of the limited size of the insect’s abdominal cavity, the high proportion of fat content results in a reduced water content. According to Su and Su (Reference Su and Su1995), the lower the moisture content, the lower the supercooling and freezing points of diapause insects at lower temperatures, and the stronger their cold resistance. However, the temperature in October was well above 0 °C in Yuxi city (Supplementary Material, Fig. S1), and C. chinensis didn’t need to reduce their moisture content to protect against low temperatures that month. The low water content of the C. chinensis that we observed in October is more likely caused by the high fat content at this time; as shown in Figures 1 and 2, the fat content was higher, and the water content was lower in the early stage of diapause, and as time passed, the fat was gradually consumed and the water content gradually increased. An increase in the moisture content in the late stages of diapause often indicates diapause cessation (Gill et al. Reference Gill, Goyal and Chahil2017). The high moisture content of C. chinensis during the post-diapause development period (May 2022) may be related to the onset of adult feeding.
The lipids stored by diapause insects often accumulate before the onset of diapause to cope with adversities such as low temperature and food scarcity. As diapause progresses and metabolic needs arise during diapause, lipids are converted into other substances to ensure the insects’ survival (Michaud and Denlinger Reference Michaud and Denlinger2006; Vukašinović et al. Reference Vukašinović, Pond, Worland, Kojić, Purać, Popović and Grubor-Lajšić2015; Ren et al. Reference Ren, Qi, An, Han and Chen2016). In the present study, the fat content of C. chinensis was found to gradually decline over time: the fat content at the start of diapause (October 2021) was 3.9 times that during the post-diapause development period (Fig. 2A). Ren et al. (Reference Ren, Zhang, Qi, An and Han2015) determined the fat content of Coccinella septempunctata (Coleoptera: Coccinellidae) at different stages and found that the abdomen of diapause adults was enriched with abundant fat bodies, with a fat content of 173.66 ± 19.01 mg/g, which was 2.2 times that of nondiapause individuals. This result is similar to the results of the present study. Moreover, Zhang’s (Reference Zhang2025) anatomical findings of male and female adult C. chinensis during diapause and post-diapause development periods showed that fat bodies occupy almost the entire abdominal cavity in the early and middle stages of diapause, but during the post-diapause development period, the fat bodies become rare or almost invisible in the abdominal cavity, which also indicates that the fat content of reproductive diapause (adult diapause) insects is gradually decreasing. Compared with lipids, glycogen is a direct source of energy for diapause insects, whereas trehalose is a blood carbohydrate and the main transported form of carbohydrate in insects (Wang Reference Wang2001). Trehalose also serves as a cold-resistant substance for overwintering insects (Qin et al. Reference Qin, Luo, He and Wu2015), and both glycogen and trehalose convert into each other (Wang and Li Reference Wang and Li2002). The present study found inconsistent changes in the glycogen and trehalose contents of C. chinensis during the diapause (from October 2021 to April 2022) and post-diapause development periods (May 2022). The glycogen content remained at lower levels during diapause but rose sharply during the post-diapause development period, becoming significantly higher than during diapause (Fig. 3A), and the glycogen content of C. chinensis during diapause remained at lower levels, probably because C. chinensis inhibits metabolism and respiration during diapause. After diapause is initiated, glycogen is substantially converted into sorbitol and glycerol, which are resynthesised into glycogen in the post-diapause development period (Chino Reference Chino1957; Kihara et al. Reference Kihara, Itoh, Iwasaka, Niimi, Yamashita and Yaginuma2009). In addition, C. chinensis migrate from the overwintering site back to the host plant and start feeding in May, which may contribute to a lower glycogen content during diapause and a rapid increase in glycogen content in May.
Changes in trehalose content were more complex: it gradually declined in the early stages of diapause (from October to December 2021), increased significantly in the middle stages (January 2022), declined gradually in the late stages (from February to April 2022), and then increase significantly again during the post-diapause development period (May 2022; Fig. 4A). Trehalose provides both energy and protection from cold (Elbein et al. Reference Elbein, Pan, Pastuszak and Carroll2003). The insects feeding before migration contributed to the large accumulation of trehalose in C. chinensis in the early stages of diapause (October 2021), with the trehalose then being gradually consumed in November and December. The lower temperatures experienced in January appeared to induce rapid synthesis of trehalose (Overgaard et al. Reference Overgaard, Malmendal, Sørensen, Bundy, Loeschcke, Nielsen and Holmstrup2007; Xie et al. Reference Xie, Xu, Zhao, Li, Qin and Xiao2023; Zhang et al. Reference Zhang, Qi, Chen, Li, Hu and Wang2023), which might have contributed to the increase in trehalose content in that month. Moreover, low-temperature stimulation contributes to the termination of diapause in insects (Morgan and Chippendale Reference Morgan and Chippendale1983; Li Reference Li2011); in the present study, January 2022’s lower temperatures might have triggered a gradual transition from the diapause maintenance to the post-diapause quiescent stage in C. chinensis. One possible reason why the trehalose content of males was found to be higher than that of females in January, April, and May 2022 is that males respond earlier to the post-diapause quiescent stage (from January to April 2022) than females do (Zhang Reference Zhang2025). This instance of asynchrony between C. chinensis males and females may be related to males replenishing their energy earlier in the post-diapause development period so as to be fit and ready to actively seek females to mate with as soon as the females exit diapause. Future studies are recommended to verify and confirm our results.
At present, glycogen and trehalose are the two main types of carbohydrate known to accumulate in diapause insects (Hayakawa and Chino Reference Hayakawa and Chino1982). Adults of C. septempunctata achieve carbohydrate accumulation during diapause by accumulating large amounts of glycogen (Ren et al. Reference Ren, Zhang, Qi, An and Han2015). By contrast, in Aphidius gifuensis (Hymenoptera: Braconidae), trehalose content increases during diapause while glycogen content decreases, suggesting that diapausing A. gifuensis obtain carbohydrates by accumulating trehalose (Li Reference Li2011). In the present study, C. chinensis maintained significantly higher levels of trehalose than that of glycogen during diapause: by the beginning of diapause (October 2021), the insect had accumulated large amounts of trehalose, which was consumed in the early stages of diapause (from October to December 2021) and then was largely accumulated again in January. Clearly, the carbohydrate accumulated in C. chinensis for diapause is trehalose.
The concentration of free amino acids in insect haemolymph is relatively high during diapause (Hahn and Denlinger Reference Hahn and Denlinger2011). These amino acids can serve as metabolic intermediates for the anabolism and catabolism processes of insects between the diapause and post-diapause development periods, such as the folding of active proteins and the recovery of development during post-diapause development period (Morgan and Chippendale Reference Morgan and Chippendale1983; Hahn and Denlinger Reference Hahn and Denlinger2011; Denlinger et al. Reference Denlinger, Yocum, Rinehart and Gilbert2012). The amino acids can also regulate the osmotic pressure of insect haemolymph to enhance insects’ cold resistance. Diapause insects generally store amino acids by accumulating special storage proteins, the accumulation of which starts before insects enter diapause. Insects continuously synthesise these proteins during diapause, and the accumulated proteins rapidly disappear once the insects enter their post-diapause development period (Hahn and Denlinger Reference Hahn and Denlinger2007, Reference Hahn and Denlinger2011). The concentration of these proteins is influenced by factors such as diapause state, oxygen, and temperature (Rivers et al. Reference Rivers, Lee and Denlinger2000; Goto et al. Reference Goto, Sekine, Outa, Hujikura and Suzuki2001). The present study determined that the protein content levels in C. chinensis were low in the early stages of diapause (from October to December 2021) – significantly lower than levels in the middle and late stages of diapause (from January to April 2022) and during the post-diapause development period (May 2022). Protein content rose sharply in January 2022 and remained relatively high until May (Fig. 5A). Average protein content from January to May 2022 was 7.3 times that in the early stage of diapause (from October to December 2021). The sharp rise in protein content in January may be closely related to local temperature and diapause state because January is the coldest month of the year in the Yuxi region: over the past decade, the lowest temperature and average temperature in January were 3.03 ± 1.27 °C and 9.02 ± 1.18 °C, respectively (China Meteorological Administration 2022). This means that C. chinensis may need to accumulate a large amount of proteins to survive the cold in January. Moreover, studies on other insects have shown low-temperature stimulation contributes to the termination of diapause in insects (Higaki and Ando Reference Higaki and Ando2005; Li et al. Reference Li, Zhou, Shi, Yao, Liao and Ting2018). In the present study, protein content in C. chinensis rose sharply in the middle and late stages of diapause (from January to April 2022), after which it remained at a relatively higher level. This may indicate that, from January 2022, C. chinensis experienced a gradual transition from diapause maintenance to the post-diapause quiescent stage. Zhang (Reference Zhang2025) confirmed that the reproductive systems of overwintering adults collected from mid-January 2024 develop significantly after the insects are exposed to favourable conditions (25 °C, 15:9-hour light:dark photoperiod, and 70% relative humidity) for 12 days, whereas no changes were observed in adults collected every 15 days in August–December 2023 under the same conditions.
A similar study (Wu et al. Reference Wu, Zhou, Zhao, Jin and Gou2019) was also conducted in the population of C. chinensis in Xijiu Town, Zunyi, Guizhou, China (28° 09′ N, 106° 10′ E; altitude: 328 m). The fat content of this geographic population during diapause was similar to that observed in the present study, except that the changes observed in the in the Xijiu-area C. chinensis carbohydrate (glycogen and trehalose) and protein content levels during diapause differed significantly. Due to significant latitude gradients in climatic conditions (such as temperature and day length), significant differences in diapause characteristics between populations residing at different latitudes can occur (Danks Reference Danks1987; Tyukmaeva et al. Reference Tyukmaeva, Lankinen, Kinnunen, Kauranen and Hoikkala2020). For example, on account of latitude-driven geographical variations in the critical photoperiod that induces diapause (Tauber et al. Reference Tauber, Tauber and Masaki1986; Danks Reference Danks1987), the diapause intensity of some insects is negatively correlated with latitude gradients; that is, the higher the latitude, the lower the diapause intensity (Masaki Reference Masaki1999, Reference Masaki2002). The physiological and biochemical characteristics of insects during diapause also vary greatly with latitude. For example, Duan (Reference Duan2015) found no significant correlation between the moisture content of Ectropis obliqua (Lepidoptera: Geometridae) and change in latitude, but the insect’s fat, protein, and glycogen contents increased with latitude; notably, its cold resistance also tended to be enhanced with latitude.
By investigating changes in the moisture, fat, carbohydrate, and protein content of C. chinensis between the diapause and post-diapause development periods, the present study has provided preliminary clarification of the dynamic changes in the physiological characteristics of C. chinensis between the diapause and post-diapause development periods, providing a scientific basis for further research on the diapause physiology of C. chinensis. Further research on the accumulation, conversion, and regulation of nutrients in C. chinensis during diapause is recommended to increase understanding of the physiological mechanisms underlying diapause of C. chinensis.
Supplementary material
The supplementary material for this article can be found at https://doi.org/10.4039/tce.2025.10022.
Data availability statement
All data supporting the findings of this study are available within the article. Source data are provided with this paper after publication.
Acknowledgements
This work was supported by XD (Xingdian) Talent Support Program, the Scientific Research Fund project of Education Department of Yunnan Province (2022J0758), the Science and Technology Program of Yunnan Province (202301AU070134), and the Special Basic Cooperative Research Programs of Yunnan Provincial Undergraduate Universities’ Association (202301BA070001-086).
Author contributions
Z.C. and S.Y. designed the experiment and wrote the manuscript. C.Z. and K.G. performed the experiment and data analysis; they contributed equally to the paper.
Competing interests
The authors declare that they have no competing or financial interests.



