





Introduction
Mistletoes are key drivers of ecological processes in terrestrial ecosystems, shaping plant community structure, biodiversity, and ecosystem functioning (Press and Phoenix Reference Press and Phoenix2005; Watson Reference Watson2001, Reference Watson2016). In savanna woodland ecosystems, they provide food and habitat for diverse fauna including birds, insects, and mammals while modifying nutrient cycling and litter dynamics (Ndagurwa et al. Reference Ndagurwa, Dube and Mlambo2013, Reference Ndagurwa, Dube and Mlambo2014, Reference Ndagurwa, Nyawo and Muvengwi2016a, Reference Ndagurwa, Ndarevani, Muvengwi and Maponga2016b). Despite their typically low abundance, mistletoes exert disproportionately large effects on these processes, positioning them as keystone species or ecosystem engineers (Watson Reference Watson2001).
Mistletoes are obligate hemiparasitic plants that attach to host trees and shrubs, extracting water, mineral nutrients, and organic compounds through specialised haustorial connections (Ehleringer et al. Reference Ehleringer, Schulze, Ziegler, Lange, Farquhar and Cowar1985; Griebel et al. Reference Griebel, Watson and Pendall2017). Because mistletoes are strong physiological sinks, infected hosts experience chronic water stress, altered nutrient allocation, and reduced carbon balance, constraining resource availability for host growth and reproduction (Ehleringer et al. Reference Ehleringer, Schulze, Ziegler, Lange, Farquhar and Cowar1985). The physiological stress also increases susceptibility to pests, diseases, and environmental stressors (Griebel et al. Reference Griebel, Watson and Pendall2017; Watson et al. Reference Watson, McLellan and Fontúrbel2022). Although the magnitude of these effects varies with infection intensity, host species, and environmental conditions (Mellado and Zamora Reference Mellado and Zamora2020; Press and Phoenix Reference Press and Phoenix2005), they are particularly severe under semi-arid conditions where water and minerals are limiting (Daneshvar et al. Reference Daneshvar, Tigabu, Karimidoost, Farhadi and Odén2014; Maponga Reference Maponga2021; Ndagurwa Reference Ndagurwa2015).
The physiological costs of mistletoe infection can extend beyond individual hosts to influence population dynamics through their effects on reproduction and recruitment (Mathiasen et al. Reference Mathiasen, Nickrent, Shaw and Watson2008; Mellado and Zamora Reference Mellado and Zamora2020; Press and Phoenix Reference Press and Phoenix2005). Mistletoe infection constrains reproduction and recruitment by creating resource stress that limits flowering, fruit development, and seed production (Arruda et al. Reference Arruda, Fadini, Carvalho, Del-Claro, Mourão, Jacobi, Teodoro, Berg, Caires and Dettke2012; Cruz Neto et al. Reference Cruz Neto, Leal, Santos and Lopes2017; Daneshvar et al. Reference Daneshvar, Tigabu, Karimidoost, Farhadi and Odén2014). Consequently, although some species exhibit compensatory reproductive responses, resource stress associated with mistletoe infection constrains reproductive output through increased flower and fruit abortion and reduced seed production, which ultimately lowers soil seedbank densities (Baskin and Baskin Reference Baskin and Baskin2014; Obeso Reference Obeso2002). In savanna ecosystems, soil seedbanks are critical reservoirs of propagules that facilitate recruitment during favourable periods when water availability and fire regimes permit establishment (Skoglund Reference Skoglund1992). Depleted seedbanks consequently reduce regeneration potential during favourable recruitment periods, leading to fewer seedlings entering the population and a shift toward older, larger individuals, thereby influencing woody vegetation abundance and demographic structure (Skoglund Reference Skoglund1992). Therefore, by constraining both reproductive output and seedbank replenishment, mistletoe infection can influence recruitment dynamics, population demography, and long-term woodland persistence and structure (Mellado and Zamora Reference Mellado and Zamora2020; Watson Reference Watson2001, Reference Watson2016). Despite extensive documentation of mistletoe effects on host physiology and growth, relatively little research addresses impacts on host reproductive performance, particularly in African savanna systems (Maponga Reference Maponga2021).
Therefore, we investigated the influence of mistletoe infection on the reproductive performance of Vachellia karroo, a widespread and ecologically important tree in southern African savannas (Barnes et al. Reference Barnes, Filer and Milton1997; Ndagurwa and Dube Reference Ndagurwa and Dube2013a, Reference Ndagurwa and Dube2013b). Specifically, the number of flower buds, number of flowers, number of pods, pod length, pod diameter, pod width, number of seeds per pod, and soil seedbank abundance were quantified to assess the effect of mistletoe infection on host reproductive output. We hypothesised that mistletoe infection reduces reproductive allocation due to competition for water, nutrients, and photosynthates. By linking parasitic stress to multiple stages of reproduction, this study contributes to a mechanistic understanding of host–parasite interactions and their implications for woody plant population dynamics and regeneration in semi-arid savannas.
Materials and methods
The study was conducted in a 160 ha woodland at the National University of Science and Technology in the southwestern highveld of Zimbabwe (20°08′S, 28°36′E). The site is fenced, with occasional firewood collection for domestic use, and veld fires are actively suppressed. Climate is strongly seasonal, comprising a hot wet season (November–April), a cool dry season (May–July), and a hot dry season (August–October). Mean annual rainfall is approximately 600 mm (range: 325–915 mm), with periodic droughts, and mean annual temperature is 23.7°C. Soils are predominantly shallow, sandy, loamy, siallitic soils derived from granite (Nyamapfene Reference Nyamapfene1991). Vegetation is deciduous, open savanna woodland adapted to semi-arid conditions and occasional frost. Colophospermum mopane (Kirk ex Benth.) Kirk ex J. Leonard, Vachellia karroo Hayne, Vachellia nilotica (L.) Willd. Ex Delile, Vachellia gerrardii Benth., and Dichrostachys cinerea (L.) Wight & Arn are dominant. Dominant grasses include Chloris virgata Swartz, Dactyloctenium aegyptium (L.) Willd., Heteropogon contortus (L.) P. Beauv. ex Roem. & Schult., Panicum maximum Jacq., Urochloa mosambicensis (Hack.) Dandy, Setaria spp., and Aristida spp. (Ndagurwa et al. Reference Ndagurwa, Ndarevani, Muvengwi and Maponga2016b). Termite mounds and mistletoes (e.g., Erianthemum ngamicum (Sprague) Danser (Loranthaceae), Plicosepalus kalachariensis (Schinz) Danser (Loranthaceae), and Viscum verrucosum Harv. (Viscaceae)) contribute to spatial heterogeneity in the site (Ndagurwa et al. Reference Ndagurwa, Ndarevani, Muvengwi and Maponga2016b, Reference Ndagurwa, Dube, Nzuma, Maponga and Muvengwi2018).
Large, canopy-dominant mistletoe-infected and uninfected V. karroo trees (n = 60 in each category) were surveyed in the woodland from December 2024 to May 2025. Then for each tree, we recorded the: (i) number of mistletoes in the canopy, (ii) height of each tree (to the nearest 10 cm) using a 10-m graduated aluminium pole, (iii) diameter at breast height (dbh) for host trees using a forest calliper, (iv) length of the long (D
1) and short (90° of D
1; = D
2) diameters of the canopy using a tape measure (to the nearest 10 cm), and the canopy area (m2) was calculated as
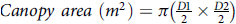 $\textit{Canopy area}\ \left(m^{2}\right)=\pi \left({D1 \over 2}\times {D2 \over 2}\right)$
.
Each tree was divided into four quadrants using the cardinal directions (N, E, W, S), within which the number of flower buds, number of flowers, number of pods, pod length, pod width, pod diameter, seeds per pod, and seed bank abundance were recorded. Flower buds and flowers were counted in December 2024, coinciding with the peak flowering period. Pod counts were conducted between March and May 2025, with each tree assessed on three occasions. During each sampling event, pods were counted twice and the mean value used for analysis (Walters and Milton Reference Walters and Milton2003). Approximately ±50 dehisced pods were randomly collected from the canopy of each tree. Pod diameter, width, and length were measured, and the number of seeds per pod recorded. Soil seedbank samples were collected at half the distance between the tree bole and the canopy edge using a steel quadrat (0.3 m × 0.3 m, 10 cm depth) (Maponga Reference Maponga2021). The four samples per tree were pooled, sieved (2 mm) to extract V. karroo seeds, and counted on a white background under high light. Sampling was conducted between May and August 2025, prior to seed release.
To assess the effects of mistletoe infection on host tree reproductive performance, generalised linear models implemented in the stats package were fitted separately for each response variable: number of flower buds, number of flowers, number of pods, seed bank abundance, pod length, pod width, pod diameter, and seeds per pod. Predictor variables included infection status (infected or uninfected), tree height (m), diameter at breast height (cm), canopy area (m2), and mistletoe abundance. To determine whether the effects of host tree size varied with infection intensity, interaction terms between mistletoe abundance and each tree size variable (height × number of mistletoes, diameter × number of mistletoes, and canopy area × number of mistletoes) were included in the models.
Prior to analysis, multicollinearity among predictor variables was assessed using variance inflation factors (VIFs) using the car package (Fox and Weisberg Reference Fox and Weisberg2019), and predictors with VIF values <5 were considered acceptable. Model assumptions were evaluated by inspecting residual plots and testing for normality and homoscedasticity of residuals. Standardised regression coefficients were calculated to facilitate comparison of effect sizes among predictors. To account for multiple comparisons across model parameters, p-values were adjusted using the Benjamini–Hochberg false discovery rate procedure (Benjamini and Hochberg Reference Benjamini and Hochberg1995). Model performance was assessed using adjusted coefficients of determination (adjusted R 2) and overall model significance using the parameters package (Lüdecke et al. Reference Lüdecke, Ben-Shachar, Patil, Waggoner and Makowski2020). The fitted models were visualised using partial effects plots and interaction plots showing model predictions with 95% confidence intervals using ggplot2 (Wickham Reference Wickham2016). All analyses were conducted in R (version 4.6.0, R Core Team 2026).
Results
Mistletoe abundance reduced bud production, pod length, pod width, pod diameter and seeds per pod (Figure 1; Table S1). Uninfected trees produced greater pod length, diameter, and width than mistletoe-infected trees (Table S1).
Partial effects of tree height and mistletoe abundance on reproductive traits of Vachellia karroo. Lines represent model predictions from generalised linear models, with shaded areas showing 95% confidence intervals while holding all other predictors constant.

Figure 1. Long description
The image contains eight scatter plots arranged in a 2x4 grid, each showing the relationship between mistletoe abundance or tree height and different reproductive traits of Vachellia karroo. Panel A: The scatter plot shows the relationship between the number of mistletoes and the number of flower buds. The x-axis represents mistletoes, and the y-axis represents flower buds. There is a negative trend, indicating that as the number of mistletoes increases, the number of flower buds decreases. Panel B: The scatter plot shows the relationship between the number of mistletoes and pod length. The x-axis represents mistletoes, and the y-axis represents pod length. There is a slight negative trend, indicating a minor decrease in pod length with an increase in mistletoes. Panel C: The scatter plot shows the relationship between the number of mistletoes and pod width. The x-axis represents mistletoes, and the y-axis represents pod width. There is a slight negative trend, indicating a minor decrease in pod width with an increase in mistletoes. Panel D: The scatter plot shows the relationship between the number of mistletoes and pod diameter. The x-axis represents mistletoes, and the y-axis represents pod diameter. There is a negative trend, indicating that as the number of mistletoes increases, the pod diameter decreases. Panel E: The scatter plot shows the relationship between the number of mistletoes and the number of seeds. The x-axis represents mistletoes, and the y-axis represents seeds. There is a slight negative trend, indicating a minor decrease in the number of seeds with an increase in mistletoes. Panel F: The scatter plot shows the relationship between tree height and the number of flower buds. The x-axis represents height, and the y-axis represents flower buds. There is a positive trend, indicating that as tree height increases, the number of flower buds increases. Panel G: The scatter plot shows the relationship between tree height and pod width. The x-axis represents height, and the y-axis represents pod width. There is a positive trend, indicating that as tree height increases, pod width increases. Panel H: The scatter plot shows the relationship between tree height and pod diameter. The x-axis represents height, and the y-axis represents pod diameter. There is a positive trend, indicating that as tree height increases, pod diameter increases. Each plot includes model predictions represented by lines, with shaded areas showing 95% confidence intervals while holding all other predictors constant.
Increasing tree diameter was associated with significant reductions in seed bank abundance, pod length, pod width, pod diameter, and seeds per pod (Fig. S1; Table S1). In contrast, canopy area exhibited positive relationships with all reproductive variables, with larger-canopy trees producing greater seed bank abundance, longer and larger pods, and more seeds per pod (Fig. S1). Host tree height also positively influenced flower bud production, pod width, and pod diameter (Figure 1).
Interaction plots revealed that mistletoe abundance altered how host tree size affected reproductive traits. The strongest interactions occurred under high mistletoe loads (75th percentile), where tree size relationships diverged markedly from low and moderate infection levels (Table S1; Figure 2). Increasing tree diameter produced opposite effects depending on infection severity. In heavily infected trees, larger diameter was associated with pronounced declines in pod width, pod length, and seed production. In contrast, lightly infected trees showed minimal changes in these traits across diameter ranges (Figure 2). Reproductive responses to canopy area followed the opposite pattern: they increased more rapidly in heavily infected trees than in lightly infected trees (Figure 2). Reproductive traits declined slightly with height at low mistletoe abundance, but increased under high mistletoe abundance (Figure 2). In contrast, seed bank abundance increased with height at low mistletoe abundance, but declined under high mistletoe abundance.
Interaction effects between tree size (height, diameter, and canopy area) and mistletoe abundance on reproductive traits of Vachellia karroo. Predictions are shown for low, medium, and high mistletoe abundance (25th, 50th, and 75th percentiles, respectively), with shaded 95% confidence intervals and grey points representing observed values.

Discussion
Mistletoe abundance negatively affected flower bud production, suggesting that increasing parasitic load reduces host reproductive investment likely through resource competition (Arruda et al. Reference Arruda, Fadini, Carvalho, Del-Claro, Mourão, Jacobi, Teodoro, Berg, Caires and Dettke2012; Cruz Neto et al. Reference Cruz Neto, Leal, Santos and Lopes2017; Daneshvar et al. Reference Daneshvar, Tigabu, Karimidoost, Farhadi and Odén2014). Mistletoes impose substantial physiological costs on their hosts by extracting water and mineral nutrients, thereby reducing resources available for reproduction (Daneshvar et al. Reference Daneshvar, Tigabu, Karimidoost, Farhadi and Odén2014; Mellado and Zamora Reference Mellado and Zamora2020; Press and Phoenix Reference Press and Phoenix2005; Silva and Martinez del Rio Reference Silva and Martinez del Rio1996). Because flowering and fruiting are energetically demanding processes, sustained resource diversion is expected to constrain reproductive effort (Obeso Reference Obeso2002). These effects are particularly severe in semi-arid savannas, where water and nutrient availability already limit plant performance. Under such conditions, mistletoe parasitism may intensify host stress and further reduce allocation to reproductive structures (Daneshvar et al. Reference Daneshvar, Tigabu, Karimidoost, Farhadi and Odén2014; Maponga Reference Maponga2021). The negative effects extended throughout the reproductive cycle, with increasing mistletoe abundance associated with reductions in pod length, width, diameter, and seed production, indicating that resource limitation persists from flowering through seed development (Daneshvar et al. Reference Daneshvar, Tigabu, Karimidoost, Farhadi and Odén2014; Maponga Reference Maponga2021; Silva and Martinez del Rio Reference Silva and Martinez del Rio1996).
Tree size emerged as a critical mediator of mistletoe impacts (Maponga Reference Maponga2021; Ndagurwa Reference Ndagurwa2015). Tree diameter was negatively associated with reproductive traits, suggesting an age- or size-related shift in resource allocation from reproduction towards maintenance and structural growth (Obeso Reference Obeso2002). In contrast, tree height and canopy area were positively related to reproductive output, indicating that larger trees possess greater resource reserves and photosynthetic capacity to support flowering and fruit production (Niklas Reference Niklas1994; Thomas Reference Thomas, Meinzer, Lachenbruch and Dawson2011). Critically, this size-dependent advantage operates differently across infection levels. Under low mistletoe loads, larger individuals can draw on greater resource pools to buffer physiological costs, while under heavy infection, this advantage becomes context-dependent as larger diameter trees also support more mistletoes and experience higher absolute resource demands, causing stronger declines in pod size and seed production (Daneshvar et al. Reference Daneshvar, Tigabu, Karimidoost, Farhadi and Odén2014; Maponga Reference Maponga2021; Silva and Martinez del Rio Reference Silva and Martinez del Rio1996). In contrast, trees with larger canopy areas show enhanced reproductive output even under high mistletoe loads, suggesting that expansive leaf area and photosynthetic capacity enable acquisition of resources sufficient to offset those extracted by mistletoes (Maponga Reference Maponga2021; Watson Reference Watson2009).
Tree height showed a critical threshold effect under parasitic stress. Height conferred minimal reproductive benefits under low mistletoe abundance, but enhanced reproductive output when parasite loads were high, implying that greater stature becomes increasingly important as parasitic stress intensifies (the host quality hypothesis; Watson Reference Watson2009). The reversal of the positive tree height–seedbank relationship under high mistletoe load indicates that increasing parasite loads can overwhelm the resource-acquisition advantages of taller trees, constraining their contribution to regeneration (Watson Reference Watson2009). Consequently, low seed bank abundance limits seedling recruitment, skewing population structure toward older, larger individuals, thereby influencing woody vegetation abundance and demographic structure (Skoglund Reference Skoglund1992).
In conclusion, mistletoe parasitism fundamentally shifts how trees allocate resources to reproduction. Small and mid-sized trees suffer disproportionate reproductive losses because they cannot generate sufficient resources to both support parasite loads and maintain flowering and fruiting. Only the largest individuals, those with expansive canopies, retain reproductive capacity under heavy infection. This creates a critical bottleneck: as mistletoe infection intensifies, only a subset of the host population contributes meaningfully to regeneration, fundamentally altering savanna population structure toward dominance by large, heavily infected adults and reducing recruitment of younger cohorts. By selectively suppressing reproduction in smaller size classes while sparing the largest trees, mistletoe infection reshapes forest demography and regeneration potential, establishing mistletoes as keystone drivers of savanna ecosystem assembly and succession (Griebel et al. Reference Griebel, Watson and Pendall2017; Mathiasen et al. Reference Mathiasen, Nickrent, Shaw and Watson2008; Ndagurwa et al. Reference Ndagurwa, Ndarevani, Muvengwi and Maponga2016b; Reference Ndagurwa, Dube, Nzuma, Maponga and Muvengwi2018; Watson Reference Watson2001, Reference Watson2016).
Supplementary material
The supplementary material for this article can be found at https://doi.org/10.1017/S0266467426100674.
Acknowledgements
Special thanks to Alford Magwizi for assistance with data collection.
Financial support
This research received no specific grant from any funding agency, commercial, or not-for-profit sectors.
Competing interests
The authors declare no competing interests.


 Open access

