1. Introduction
Neuroconstructivism draws on three traditions. The first is the constructivist view of development attributed to Piaget and his contemporaries, such as the developmental biologist Waddington. “Neuro” introduces the second tradition: a commitment to view psychological development as entwined with the mechanistic and morphological aspects of brain development, from cell to brain to body. Third is computational modeling, which forces process theories to be explicit about the nature of information processing, resulting in a level of specification that eludes traditional, verbal, descriptive theories. Two recent books brought two of these three traditions together. Rethinking innateness (Elman et al. Reference Elman, Bates, Johnson, Karmiloff-Smith, Parisi and Plunkett1996) argued for a connectionist modeling approach to understanding brain and cognitive development. In contrast, A dynamic systems approach to the development of cognition and action (Thelen & Smith Reference Thelen and Smith1994) emphasized development as occurring in the context of embodiment. In Neuroconstructivism, volume 1: How the brain constructs cognition (Mareschal et al. Reference Mareschal, Johnson, Sirois, Spratling, Thomas and Westermann2007a), we add a focus on neural development and the development of representations.
NeuroconstructivismFootnote 1 emphasizes the interrelation between brain development and cognitive development. We see constructivist development as a progressive increase in the complexity of representations, with the consequence that new competences can develop based on earlier, simpler ones. This increase in representational complexity is realized in the brain by a progressive elaboration of cortical structures. Thus, while other constructivist theories have emphasized the notion of hierarchical integration of knowledge (e.g., Karmiloff-Smith Reference Karmiloff-Smith1992; Piaget Reference Piaget1970), we explore the relationship between the elaboration of knowledge and the development of new cognitive abilities. We assert that increases in representational complexity arise as a natural consequence of the processes of adaptation typical of complex biological systems like the brain (for related views see Mareschal & Shultz Reference Mareschal and Shultz1996; Quartz & Sejnowski Reference Quartz and Sejnowski1997; Shultz Reference Shultz2003). Neuroconstructivism implies the creation of genuinely new cognitive abilities and not just the better use of preexisting abilities.
While our focus is on the development of mental representations, these develop in a physical and social environment. The body, which changes substantially during infancy, constrains what the infant can experience, process, and do. This, in turn, constrains possible learning and development. For example, the limited visual acuity of babies helps simplify the visual environment, and could also help with the integration of modalities as the clearest objects are those within reach. Physical constraints on action also force a “starting small” situation, whereby the child learns simpler effective behavior before being able to acquire more complex abilities. The social environment also constrains what and how the child will learn. The use of motherese, for instance, simplifies the linguistic input early in language acquisition. Indeed, most human societies engage in a process of gradually exposing infants and children to the kinds of problems that they will need to master in order to survive.
The guiding principle behind our approach is context dependence. Representations in the brain do not emerge or function in isolation, but within the context of cooccurring molecular, neural, bodily, and social events. This constrains and guides emerging representation through three mechanisms: cooperation, competition, and chronotopy (see section 2.4). The mechanisms take different forms at the different levels of implementation, but together they enable two central developmental processes: proactivity, which is concerned with the role of internally generated activity in the development of function, and progressive specialization, the fact that functions exhibit a progressive restriction of fate by becoming more specific and less plastic.
We argue that the outcome of these developmental mechanisms and processes are partial representations. The brain acquires and develops multiple, fragmentary representations that are just sufficient for on-the-fly processing. The role of developmental psychology is to understand how and why such partial representations emerge, how they interact, and how flexibile their configuration is.
One novel aspect of our approach is that our emphasis on context requires consistency among levels of explanation. We view cognitive functions as inextricably linked to their neural implementation and to the dynamic environments in which they emerge and operate, with interactions going both ways across levels. As far as explaining cognitive development, we see little merit in theories or models that fit data at one level, however well, yet contradict what is known at other levels. Thus, we argue for a radical rejection of Marr's (Reference Marr1982) independent levels of analysis argument. While explanations can be formulated independently at different levels of description, those levels are not themselves independent. A consequence of our focus on consistency is parsimony. If a phenomenon can be explained at different levels using a unitary framework, then this is preferable to an alternative where different and inconsistent interpretations are used at each level.
In the next section, we lay out the foundations of neuroconstructivism, culminating with a proposed set of principles, mechanisms, and processes. Section 3 illustrates these ideas through the use of case studies in which the neuroconstructivist framework is applied to different domains of cognitive development. In a concluding section, we identify future challenges and briefly discuss Neuroconstructivism, volume 2: Perspectives and prospects.
2. Foundations
2.1. Encellment
The development of the nervous system is typically described as a two-stage process. Initially, coarse structure and connectivity is laid out, with little contribution from the electrical activity of neurons. Then, the firing of neurons becomes crucial in establishing the finer-grained details of connectivity. Therefore, to examine brain development at the cellular level, we need to distinguish between context-dependent and activity-dependent processes (Crowley & Katz Reference Crowley and Katz1999; Herrmann & Shatz Reference Herrmann and Shatz1995).
In the early stages of neural development, activity probably plays the smallest of any role in the outcome. In neurogenesis, precursor cells (neuroblasts) differentiate into neurons, glial cells, or new precursor cells. The outcome of differentiation is affected both by the lineage of the cell and, crucially, by cell-cell interactions. A new neuron then migrates to its final position, either by passive displacement (i.e., being pushed by other emerging neurons) or with the help of radial glial cells that guide neural migration. Thus, local cellular context plays a key role in the formation of neural structures.
Neural differentiation begins during, or towards the end of, migration. Axons often traverse long distances (Purves et al. Reference Purves, Augustine, Fitzpatrick, Katz, LaMantia and McNamara1997), facilitated by a mixture of activity-dependent and activity-independent processes. A neurite (the neuron outgrowth that will become the axon) develops protrusions that will travel in space in response to both chemical and physical extracellular events. Particular cues guide axonal growth while others impair it, and processes can seek specific target locations with a unique chemical signature (Goodman & Shatz Reference Goodman and Shatz1993). Once in a target area, an axon forms specific connections with dendrites through competition with other dendrites and other axons. Endogenous electrical activity also plays a role in early, presynaptic neural differentiation such that early in brain development, one observes key roles for both context- and activity-dependence.
Overproduction of cells leads to programmed cell death (Oppenheim Reference Oppenheim1991). The death of a neuron is controlled by a combination of intrinsic and extrinsic factors, whereby an internal “suicide” program will be triggered or suppressed by external chemical events involved in the guidance and competition for neural differentiation through trophic factors. Crucially, neural activity appears to have a protective effect on neurons, as it reduces cell death (Ghosh et al. Reference Ghosh, Carnahan and Greenberg1994).
Activity-dependence is one part of a feedback loop with morphology, with each affecting the other. The activity of neurons can also alter subcellular ion channels and neurotransmitter receptors, so that the response profile of a neuron is adaptive over time (Turrigiano et al. Reference Turrigiano, Abbott and Marder1994). Gene expression, too, can be affected by neural activity (Armstrong & Montminy Reference Armstrong and Montminy1993). Activity-dependence also affects the connectivity between cells. A good example is the emergence of ocular dominance columns (ODCs): Preventing sensory input to one eye considerably reduces the space occupied by neurons responding to that eye, illustrating activity-dependent competition.
Two competing theories have been proposed to explain the emergence of cortical areas. One is the protomap view (Rakic Reference Rakic1988), which suggests that neurons are predestined early in development to occupy specific functions in specific cortical areas. The second is the protocortex view (O'Leary & Stanfield Reference O'Leary and Stanfield1989), which argues that functional areas emerge from interactions with subcortical structures and between cortical areas. Recent reviews propose a midway view in which patterns of gene expression create, at a coarse scale, cortical areas more suited to adopting particular functions as per the protomap view. However, a protocortex account better explains the emergence of function within those poorly spatially and functionally defined areas.
2.2. Embrainment
Embrainment refers to the view that functional areas of the brain emerge and exist within a context of connections to and from other functional areas. This contrasts with a view of functional brain development in which regions are presumed to mature in relative isolation of their context, and with the view that particular cognitive operations can be localized to individual regions in adults. In fact, there is substantial evidence that the functional properties of specific brain regions are highly constrained by their past and present interactions with neighboring areas.
For example, visual event-related potential (ERP)components of congenitally deaf people differ markedly from those of typical hearing participants and participants who became deaf after the age of four (Neville & Lawson Reference Neville and Lawson1987). Based on these findings, Neville and Lawson (Reference Neville and Lawson1987) proposed that early (but not late) lack of auditory input allowed a reallocation of resources, such that cortical areas typically involved in auditory processing were taken over, to a degree, by visual processing. Similarly, it has been shown that the visual cortex of people blind from an early age can be activated by tactile stimuli, particularly Braille reading. In both these examples, the differentiation of the cortex into areas of functional specialization results from a developmental process and is not functionally encapsulated. If the context changes during development, then so too can the function associated with a cortical area.
There are three important questions to consider when studying the etiology of brain functions. First, does development involve deterministic epigenesis or probabilistic epigenesis (Gottlieb Reference Gottlieb2007)? With the former, the assumption is a unidirectional path between gene and brain function. With the latter, the relationship between genes, structure, and function is bidirectional and dynamic. Second, is there a direct mapping between brain structure and function, and does this change over development? The third question concerns the nature of brain plasticity, and whether the degree of plasticity changes over development.
A substantial amount of research concerned with mapping brain and behavioral development has taken a maturational viewpoint, whereby emerging behaviors are construed to reflect underlying maturing functions of isolated areas of the brain (see Diamond Reference Diamond, Gibson and Petersen1991). A tacit assumption is that the typical adult brain (and thus behavior) is prespecified in a protomap (deterministic epigenesis), with a direct mapping between structure and function. Within this view, plasticity is a special mechanism activated by brain injury. An alternative to the maturational view is the skill-learning perspective, which proposes a continuity between infancy and adulthood in the mechanisms underlying brain learning and plasticity. According to this view, plasticity is a long-lasting feature of the brain that appears to be reduced only within a context of the stable constraints that are more likely in adulthood.
The interactive specialization viewpoint proposes a middle ground between the previous two accounts (Johnson Reference Johnson2005). It proposes that brain regions develop within the context of other brain regions (embrainment), and that the functional development of brain regions is shaped in part by interregional interactions. Specifically, cortical functional brain development is characterized by a process of increased tuning, or selectivity of functions. Thus, the mapping between structures and functions can and will change during development. Within this viewpoint, plasticity is retained when a function is not yet fully specialized.
Functional cortical brain development is best described as progressive localization and progressive specialization of function, through competition and cooperation between distinct areas. Representations that emerge within a region are constrained by existing representations in functionally neighboring areas, consistent with the interactive specialization view.
2.3. Embodiment
While the distinction between mind and the physical world may have surface appeal, ethological work has revealed a much closer coupling between behavior and environment. The brain is best viewed as embedded in its environment, and not divorced from it. As at other levels of organization, the study of a specific system must involve consideration of the other systems to which it is coupled. In the case of the brain, it is unhelpful to ignore the body and the external environment.
While previous work has distinguished embodiment (the constraints of the body on the brain) from situatedness (the constraints of the environment on the agent), we use embodiment to encompass both types of interaction. Taking embodiment seriously can reveal simpler solutions to cognitive problems than would be achieved by nonembodied approaches (e.g., Webb Reference Webb, Cliff, Husbands, Meyer and Wilson1994). Indeed, considering the contribution of both body and environment can reduce the purported contribution of the nervous system (Clark Reference Clark1997). For some cognitive problems, parts of the solution exist in bodily constraints and environmental properties. The role of the brain is to coordinate inner and outer worlds (Ballard et al. Reference Ballard, Hayhoe, Pook and Rao1997). Hence, representations are not independent from the environment; rather, they contain partial information about the environment, sufficient to support contextually specific behaviors. Representations serve to cause behaviors rather than to mirror the environment.
Clark (Reference Clark1997) identifies several important ways in which an embodied perspective provides benefits to cognitive research. First, it raises awareness that an important function for organisms is to harness the environment to their advantage (Hutchins Reference Hutchins1995). Second, the planning and execution of motor actions must consider body/environment couplings (Thelen et al. Reference Thelen, Corbetta and Spencer1996). Third, an embodied view stresses the online nature of information processing (Goldstein & Gigerenzer Reference Goldstein and Gigerenzer2002), which relies on context-dependent heuristics for just-in-time adaptations. Fourth, an embodied perspective recognizes how elements of the environment can act as extensions of the mind, reducing cognitive load. Fifth, Clark (Reference Clark1997) proposes that language embeds individuals within society, allowing individuals to share representations and affect one another's behavior. In terms of development, language provides a crucial tool to guide the experiences of infants and children (Rogoff Reference Rogoff and Damon1998; Vygotsky Reference Vygotsky1986).
Embodied models take one of two forms. In agent modeling, both the organism and the environment are computer simulations (e.g., Schlesinger Reference Schlesinger2004). Alternatively, researchers may use real robots that function in real environments. An example of this second approach is “Didabot” (Maris & te Boekhorst Reference Maris and te Boekhorst1996), a simple robot that avoids objects perceived by sensors on its left and right sides, near the front. The robot has a blind spot immediately in front of it. When several Didabots were placed in an enclosed environment that contained cubes small enough to fall within the robots' blind spots, the cubes ended up in heaps at the center and periphery of the arena. This apparently complex “tidying” behavior emerged from the coupling of a simple mind (avoid obstacles), body (blind spot), and environment (cubes and other robots).
Developmental embodied cognition focuses on the codevelopment of the nervous system and the body within a dynamic environment. This has roots in ecological psychology (e.g., Gibson Reference Gibson1979; Reference Gibson and Collins1982). A key concept of this earlier work is that of affordances, the fact that particular stimuli invite a specific range of actions in relation to the agent's structure and skills. Recent infancy work supports the notion of action affordance in terms of representing objects (Mareschal & Bremner Reference Mareschal, Bremner, Johnson and Munakata2005; Mareschal & Johnson Reference Mareschal and Johnson2003). Thelen and Smith (Reference Thelen and Smith1994) argued more generally that the interplay between thought and action is ubiquitous in infancy, consistent with Piaget's notion of early sensorimotor development (Piaget Reference Piaget1952). Importantly, this approach stresses how the child actively manipulates the environment, with dynamic consequences in respect to the stimulation encountered. Similarly, the onset of self-locomotion brings about such a major change in the infant's effective environment that some have argued it causes a major reorganization of cognitive structures (Campos et al. Reference Campos, Anderson, Barbu-Roth, Hubbard, Hertenstein and Witherington2000).
2.4. Principles, mechanisms, and processes
A core principle of the neuroconstructivist approach is context-dependence. At each level of description or analysis, the function of interest depends on the context in which it is realized. Furthermore, context-dependence is particularly important for the development of those functions and has significant implications for the representations that emerge.
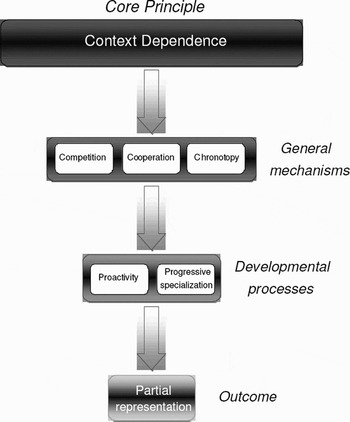
Context-dependence constrains emerging representations through three domain-general, level-independent mechanisms: cooperation, competition, and chronotopy (timing). The specific implementation of these mechanisms will vary depending on the level of analysis. The mechanisms themselves make possible two processes that underlie the development of representations: proactivity and progressive specialization. The outcome of these processes is the emergence of partial representations (Fig. 1).
Principles, mechanisms and processes involved in the neuroconstructivist framework. Both the mechanisms and processes can be construed as operating at multiple levels of description.

Competition implies that from the many initial contributors to an immature function, only a subset of these will ultimately be involved in the mature function. For example, over time, the expression of gene A may prevent the expression of gene B. Similarly, inhibitory neurons or inhibitory brain structures (e.g., frontal lobe inhibition of subcortical functions) restrict competing processes from participating in a particular function. At the cognitive level, one representation of a sensory input (e.g., one view of the ambiguous Necker cube) may compete with another incompatible interpretation of the same sensory data. Overall, the purpose of competition is to allow for stable, minimal representations.
Cooperation, however, is a mechanism involved in the integration of multiple contributors to a function. For example, some genes serve as triggers for other genes, coactivity of neurons help build circuits, different brain systems may need to be simultaneously involved in a particular function, and social behavior requires cooperation among individuals. Unlike competition, but complementary to it, cooperation strives for overall efficiency through the coordination of interrelated functions. Together, competition and cooperation help build a system that may be minimal but involves a degree of redundancy that makes it relatively robust to damage.
The notion of chronotopy stresses that time is a dimension of development (cf. Elman et al. Reference Elman, Bates, Johnson, Karmiloff-Smith, Parisi and Plunkett1996). Some patterns of gene expression are restricted to specific developmental times, some key aspects of neural development rely on sequences of events, and adaptive plasticity occurs at different times in different parts of the developing system. At a cognitive level, this translates to saying that children will solve restricted problems grounded within a limited domain before solving abstract general problems that span several domains. Perhaps the most important temporal aspect concerns restrictions to plasticity. Neural commitment means that some circuits, once wired, may be hard to alter. Processing commitment, which is linked to neural commitment, means that functions become progressively entrenched and selective, and may lose sensitivity to inputs outside their current range.
Two developmental processes operate on a larger time scale than the above mechanisms. Proactivity refers to the idea that, at least in part, representations reflect internally generated activity. For example, spontaneous neural activity helps form certain synaptic connections. Similarly, a child initiates behaviors that have effects on the environment that, in turn, affect sensory input and ensuing behavior. We view such a feedback loop, with key involvement from a proactive child, as the engine of development. There is substantial evidence that, from an early age, infants and children are selective about the information they process from the environment (Cohen Reference Cohen1972; Fantz Reference Fantz1964; Posner Reference Posner, Meyers and Kornblum1993). There is also evidence revealing a role for spontaneously generated movements on early development (Goldfield et al. Reference Goldfield, Kay and Warren1993; Robertson et al. Reference Robertson, Bacher and Huntington2001), even in utero (Prechtl Reference Prechtl, Kalverboer and Gramsbergen2001; Robertson Reference Robertson, Smotherman and Robinson1988).
The other developmental process is progressive specialization. In its simplest form, the state of the system at any given time places constraints on future states of the system. Waddington's (Reference Waddington1957) metaphor of an epigenetic landscape captures the idea well. According to Waddington, development is like a ball rolling down an uneven surface, able to take different directions as a function of its direction and inertia, and the landscape. Typical development would see most balls end up in the same general area of the landscape, and atypical development would see balls end up in different areas because of changes to initial direction, inertia, or landscape. A good example of such restriction-of-fate over time is phonological development. Although newborns can distinguish speech sounds from all human languages, the ability to discriminate nonnative speech sounds drops substantially after about six months (Stager & Werker Reference Stager and Werker1997; Trehub Reference Trehub1976). Importantly, progressive specialization does not simply limit future adaptations but can also facilitate learning. In a constructivist framework, early knowledge often provides the building blocks for further knowledge.
We argue that the outcomes of these developmental processes are partial representations. The brain contains multiple fragmentary and partial representations that are sufficient to allow successful behavior, for example, in response to a given object over a range of contexts. Each of these is able to have an independent causal effect on behavior. This view is consistent with the distributed processing that takes place in the brain and is a computationally efficient solution to representation. New representations are thus acquired in the context of existing (also fragmentary) representations, the current effective learning environment, and the current developmental state of the body.
3. Case studies
This section presents different areas of research that serve to exemplify how our approach can be applied in different domains. We use the term case study in the broad sense of a focused illustration. The first four case studies are concrete examples of how the mechanisms operate. The last three cases are concerned with the notion of interactions between the different levels of explanation.
3.1. Early visual perception
Visual information processing in adults involves distinct cortical regions (Van Essen et al. Reference Van Essen, Anderson and Felleman1992). For example, during object recognition, cortical processing begins in area V1 (the primary visual cortex) and progresses through a series of cortical regions until object identity per se is processed in the inferotemporal cortex. This portion of the visual system dealing with object recognition is known as the ventral pathway (Ungerleider & Mishkin Reference Ungerleider, Mishkin, Ingle, Goodale and Mansfield1982). Along this pathway early areas are involved in simpler tasks such as edge, contrast, or orientation detection (e.g., Hubel & Wiesel Reference Hubel and Wiesel1963), whereas later areas are involved in progressively more abstract representations (such as, ultimately, identifying an object). However, the pathway is not unidirectional but involves reciprocal connections between regions (Lamme & Roelfsema Reference Lamme and Roelfsema2000). Later processes can affect earlier ones, such that the dynamics of information processing are more important than their specific anatomical locations (Felleman & Van Essen Reference Felleman and Van Essen1991). Each cortical region is embedded in a network of other regions and processes information in this dynamic context.
Within each region there exists competition between cells, such as that occurring through lateral inhibition. This competition occurs at each stage of processing and reflects both bottom-up stimulation and top-down biases (Desimone & Duncan Reference Desimone and Duncan1995). Cooperation is also an important process in vision. To identify an object, it is necessary to group features of the visual input that belong to that object and to segment those from the background. This is achieved through an interactive process involving feedforward and feedback connections between the different cortical areas involved in object perception (Driver et al. Reference Driver, Davis, Russell, Turatto and Freeman2001). Chronotopy is also important, as the functionality of the visual system emerges from a peripheral to central ordering over time (Johnson & Vecera Reference Johnson and Vecera1996; Shrager & Johnson Reference Shrager and Johnson1996). Later-developing neurons in higher-order areas can exploit the earlier, partial representations developed in lower, peripheral regions. Representations learned at each level constrain the representational space of subsequent levels, allowing high-order regularities to be extracted (Clark & Thornton Reference Clark and Thornton1997).
The input selectivity of cells involved in visual processing can be changed through learning (Desimone Reference Desimone1996). Moreover, experience leads to a decrease in the population of cells that respond to a familiar stimulus (Rainer & Miller Reference Rainer and Miller2000). Changes in performance thus reflect changes in representations, distributed across a smaller, selective population of neurons (Karni et al. Reference Karni, Meyer, Jezzard, Adams, Turner and Ungerleider1995). Some work also reports that the cortical regions involved in a task may change as a function of expertise (Walsh et al. Reference Walsh, Ashbridge and Cowey1998), with fewer regions involved after learning than was initially the case (Petersen et al. Reference Petersen, Van Mier, Fiez and Raichle1998). This experience-dependent selectivity can enhance processing of subsets of visual inputs at the expense of other subsets. Selective attention implements a form of proactivity, whereby the child preferentially attends to some stimuli over others.
Overall, cortical regions involved in visual processing carry out contextualized intraregional competition and interregional cooperation, modulated by a degree of chronotopy that forces simpler representations to be acquired prior to progressively more complex representations. The progressive specialization at each level of processing reflects experience, which is proactive. The outcome is a set of partial representations across a complex network of cortical areas that together enable object recognition.
3.2. Infant habituation
Because of the limited perceptual and motor skills of infants, researchers have devised many indirect methods to assess cognitive abilities in infants. The most popular method is the use of looking-time data (e.g., Thorpe Reference Thorpe1956). Over the repeated presentation of stimuli, babies show a progressive decrease of interest, reflected by shorter looking times to the stimuli. They are then deemed to have habituated. However, they can show renewed interest (assessed from relatively longer looking) when presented with novel stimuli. This “novelty preference” is an example of proactive exploration of the environment. By careful manipulation of how the habitual and novel stimuli differ from each other, researchers can make claims about what infants perceive to be distinct, with implications for the nature of their underlying representations (Cashon & Cohen Reference Cashon and Cohen2000). A common approach, owing to the pioneering work of Sokolov (Reference Sokolov1963), is to suggest that a mental representation of the habitual set of stimuli is learned, and that the progressive decrease in looking time reflects an increasing match between this internal represenataion and the stimuli. Novelty preference is then taken to reflect a mismatch between the internal representation and the novel stimulus.
In accordance with our theme of consistency across levels of interpretation, Sirois and Mareschal (Reference Sirois and Mareschal2002) argued that models and theories of habituation should reflect the two key neural mechanisms that support infant habituation. First, the hippocampus is involved in selective inhibition of high-order features such as color or shape (or feature relations, such as color-plus-shape) of the habitual stimuli (Nelson Reference Nelson1995; Sokolov & Vinogradova Reference Sokolov and Vinogradova1975). Hippocampal inhibition is short-lived. Hence, given that habituation has lasting effects (Zelazo et al. Reference Zelazo, Weiss, Tarquinio, Weiss and Zelazo1991), the second neural mechanism of habituation involves long-term storage in hippocampal-related cortical areas, notably the entorhinal cortex (Nelson Reference Nelson1995).
In the Habituation, autoassociation and brain (HAB) model of infant habituation (Sirois & Mareschal Reference Sirois and Mareschal2004), hippocampal and cortical functions are both implemented by simple autoassociator networks (see Sirois Reference Sirois2004); however, they use different learning rules to implement selective inhibition and long-term storage. Both networks are coupled through reciprocal connections and both contribute to the overall output of the system. Embedding the model in a robot and an environment illustrated how motor learning contributes to habituation performance (Sirois Reference Sirois2005).
The HAB model illustrates the main principles of the neuroconstructivist approach in the following ways. First, learning is driven by context, as each subsystem learns within the feedback loop of the other, antagonist subsystem. Moreover, as the robot work illustrated, habituation can be affected by motor learning. Behavior involves a mixture of cooperation (within subsystems, but also between them when their outputs are aggregated at the system level) and competition (the hippocampus attempts to shut down known input signals, whereas the cortex attempts to amplify them). Moreover, chronotopy was shown by the model's ability to capture age-related changes in performance through maturation of outward connections from the cortex (Sirois & Mareschal Reference Sirois and Mareschal2004), as observed in infant brains and in absence of prior experience. The model is proactive, as it seeks maximally stimulating input (Sirois Reference Sirois2005), and exhibits progressive specialization as it shifts from an initial familiarity preference to a novelty preference once known inputs are well learned. The outcome is partial representations, as the behavior of the model is achieved through the activity of several interconnected units in two distinct subsystems.
3.3. Phonological development
Infant babbling, the repetition of simple speech sounds, creates a coupling between the perception and production of language. This view is relatively recent, as early work on phonological development proposed no such connection between babbling and speech (Jakobson Reference Jakobson and Keiler1941; Lenneberg Reference Lenneberg1967).
In the first year of life, there are substantial changes to the perception of speech sounds. The best known is how infants, who are initially able to discriminate speech sounds from any human language (Eimas et al. Reference Eimas, Siqueland, Jusczyk and Vigorito1971), progressively lose the ability to discriminate phonemes from outside their native language in the second half of the first year (Werker & Tees Reference Werker and Tees1984). The importance of the linguistic environment is further stressed by data showing that infants' speech discrimination ability is correlated with the clarity of their mothers' speech (Liu et al. Reference Liu, Kuhl and Tsao2003).
Changes in speech-sound production can be observed in infant articulation. Before six months, most speech sounds consist of isolated vowels. However, around six months, most infants begin to babble. Articulation becomes progressively more complex over the next few months, and babbling becomes more specific to the infant's native language (Boysson-Bardies et al. Reference Boysson-Bardies, Halle, Sagart and Durand1989). This is arguably a key step towards the development of a phonological inventory, used for words and subsequently more complex linguistic structures (Vihman Reference Vihman, Stamenov and Gallese2002).
The central role of auditory perception for babbling has been emphasized by research on deaf infants (Oller & Eilers Reference Oller and Eilers1988), who babble later than hearing infants and produce different sounds. These effects are long lasting and can negatively affect later speech (Wallace et al. Reference Wallace, Menn and Yoshinaga-Itano1998). Auditory feedback is thus necessary for the successful coordination of phonatory (larynx) and articulatory (vocal tract) speech systems, essential for babbling and, subsequently, speech (Koopmans-van Beinum et al. Reference Koopmans-van Beinum, Clement and van den Dikkenberg-Pot2001).
Westermann and Miranda (Reference Westermann and Miranda2004) recently proposed a mechanistic model of the development of the link between speech perception and production. The model consists of two topographic maps, one each for articulation and perception. Within these maps, neurons responded to inputs that fell within their respective fields. The two maps were connected with Hebbian weights, such that units with high covariation between maps saw their connections strengthened and connections for units with low covariation were weakened. As a consequence, strongly covarying articulations/perceptions became prototypical; these prototypes represented vowels that could be most robustly produced based on articulatory parameters. The model's prototypical speech sounds reflected both internally generated activity and environmental input (see Vihman Reference Vihman, Mattingly and Studdert-Kennedy1991 for a similar interpretation called the articulatory filter hypothesis).
Context is central to the emergence of speech sound prototypes in both maps. Articulatory representations emerge from a dynamic interaction with perception and vice versa; moreover, these reflect the context of both internally generated and external inputs. Each topographical map implements local competition through lateral inhibition, but the coupling of articulation and perception requires the cooperation of both maps. Chronotopy is also important, as both maps require a synchronization of plasticity. Proactivity is vital, as babbling produces the coupling between perception and production. Moreover, as this coupling develops, the representations make the model progressively more selective with respect to environmental input. In real infants, in a real linguistic environment, this would lead to enhanced performance in the native language, at the expense of discrimination abilities for other languages (see also McClelland et al. Reference McClelland, Fieza and McCandliss2002). Ultimately, this progressive specialization within and between maps leads to partial representations: speech sounds become activations patterns on both maps, and these cannot be isolated from one another.
3.4. Object representations in infants
Ungerleider and Mishkin (Reference Ungerleider, Mishkin, Ingle, Goodale and Mansfield1982) proposed that object processing involves two separate cortical information processing pathways: the dorsal and ventral streams. It was proposed that the dorsal stream, terminating in the parietal cortex, processes object localization (the where function), whereas the ventral system, ending in the temporal cortex, performs object identification (the what function). The actual degree of independence of these two streams has recently been the object of some attention (Fellman & Van Essen Reference Felleman and Van Essen1991; Humphreys & Riddoch Reference Humphreys and Riddoch2003; Merigan & Maunsell Reference Merigan and Maunsell1993; Puce et al. Reference Puce, Allison, Bentin, Gore and McCarthy1998). Our interest, though, is that both streams process different types of information and, as such, develop distinct representations.
The fact that object representations are, to a large degree, segregated in functionally distinct routes, implies that there needs to be a mechanism that integrates these two sources of information when they are required by some task (such as, for example, picking up a specific object from several alternatives). Mareschal et al. (Reference Mareschal, Plunkett and Harris1999) proposed a model that examines how these two streams of information may be gradually integrated over the course of development, explaining why successful object retrieval by infants lags behind successful visual tracking. A key assumption of the model is that both routes (ventral and dorsal) are exposed to the same input but differ in their associative learning mechanisms. The object recognition network (ventral stream) generates a spatially invariant representation of objects, using an unsupervised competitive learning rule (Foldiak Reference Foldiak1991). The trajectory prediction network (dorsal stream) uses a partially recurrent feedforward network to track the immediately anticipated retinal position of moving objects, a proactive process. The response integration network in Mareschal et al. (Reference Mareschal, Plunkett and Harris1999) represents a measure of infants' abilities to coordinate and use information about the positions and identities of objects, analogous to a similar prefrontal cortical function observed in primates (Rao et al. Reference Rao, Rainer and Miller1997).
Interestingly, young infants show some unusual behaviors when objects are briefly occluded. For instance, infants can remember spatial properties of occluded objects but not necessarily identity features (Kaldy & Sigala Reference Kaldy and Sigala2004; Leslie et al. Reference Leslie, Xu, Tremoulet and Scholl1998; Simon et al. Reference Simon, Hespos and Rochat1995; Wilcox & Schweinle Reference Wilcox and Schweinle2002; Xu & Carey Reference Xu and Carey1996). Object individuation at 4.5 months relies on shape and size, at 7.5 months on texture, and only at 11.5 months does it involve color (Wilcox Reference Wilcox1999). Mareschal and Johnson (Reference Mareschal and Johnson2003) examined under which conditions four-month-olds would retain position or identity information during a 5-second occlusion. They found that the functional value of objects (their affordance, in Gibsonian terms) appears to drive a competition between dorsal and ventral streams for object retention. Objects that afford the possibility of actions maintain dorsally processed information, whereas objects that do not afford action maintain ventral information.
This and other evidence highlights the contextual nature of object processing, involving the child, the environment, the affordance of objects and functionally distinct neural representations. Competition and cooperation occur at different levels in the distributed system involved in object recognition. The system also exhibits progressive specialization, in that each stream excludes irrelevant sources of information (spatial or featural) to carry out its function. Ultimately, the infant brain must coordinate partial representations in distinct systems to act on specific objects (Mareschal et al. Reference Mareschal, Plunkett and Harris1999; Rao et al. Reference Rao, Rainer and Miller1997).
3.5. Ensocialment
The importance of the social context on cognitive development has a long history (e.g., Bandura Reference Bandura1986; Rogoff Reference Rogoff1990; Vygotsky Reference Vygotsky1978). Our focus is on the developing child situated in an environment that includes other humans and in which development involves a collaboration between the child and those who support and nurture this development (Rogoff Reference Rogoff2003). While these ideas are not new, it is only more recently that the importance of social behavior has made forays into the neurosciences (e.g., Adolphs Reference Adolphs2003).
An early aspect of social brain function is the preference of newborns (as early as within the first hours after birth) for face-like stimuli (Johnson et al. Reference Johnson, Dziurawiec, Ellis and Morton1991; Valenza et al. Reference Valenza, Simion, Cassia and Umilta1996). Although the specific cues that elicit the preference remain a source of debate (see Johnson Reference Johnson2005 for review), it has been suggested that three high-contrast blobs in the positions of the eyes and mouth may be sufficient (Johnson & Morton Reference Johnson and Morton1991; Morton & Johnson Reference Morton and Johnson1991). Hence, the brain does not contain, from birth, a detailed specification of a face but a skeletal, partial, representation. The preference for face-like stimulation makes the infant proactive in seeking stimulation with faces, which places the infant in a learning context in which other cortical systems will learn about faces. Hence, an initial bias ensures that later developing areas of the cortex acquire specific specialization for faces (Johnson Reference Johnson2005). Similarly, evidence shows that infants prefer to look at faces that show direct gaze towards them (Farroni et al. Reference Farroni, Csibra, Simion and Johnson2002). Maintaining eye contact with someone ensures foveation of the face, which may prove essential to the emergence of a cortical face area (Johnson Reference Johnson, Kanwisher and Duncan2004).
Children benefit from “ensocialment” in several other ways. For example, Vygotsky (Reference Vygotsky1978) was probably the first to fully recognize the role of language in shaping cognitive development. Vygotsky argued that, cognitive change involved moving from external speech, which instructs the child, to private speech, whereby the child maintains an internal dialog that takes over from external instruction to guide behavior. Indeed, Berk and Gavin (Reference Berk and Gavin1984) observed that most vocalized private speech in group settings actually takes place when a child is working alone on a difficult task.
Vygotsky (Reference Vygotsky1978) further proposed that in relation to the child's current level of development, there existed a small window of optimal stimulation within which to provoke further development: the zone of proximal development (ZPD). Infants display this spontaneously by exhibiting a preference for stimuli that are moderately discrepant from their current knowledge or capabilities (McCall et al. Reference McCall, Kennedy and Applebaum1977). Teaching below this zone provides little enhancement as it is within the child's current grasp. Similarly, teaching above this zone would also provide few gains as the child would fail to see the path between her current level of competence and the teaching. Thus, Rogoff (Reference Rogoff1990) proposed the notion of guided participation, whereby progress is optimal when child and teacher share a focus and purpose in learning. The main idea in terms of instruction (and, generally, pedagogy) is that it channels the child's interaction with the environment (see also Csibra & Gergely Reference Csibra, Gergely, Johnson and Munakata2006). The emphasis on joint participation once again highlights the importance of proactivity from the child.
3.6. Atypical development
In most cases, the outcome of development is relatively predictable. However, how can we explain variability in developmental outcome? Some variability is observed in intelligence, much more in cases of developmental disorders. Developmental disorders can have several causes. Disorders can stem from genetic abnormalities, such as in Down syndrome, Williams syndrome, and fragile X. They can be identified on behavioral grounds, such as in autism, Specific Language Impairment (SLI), Attention Deficit Hyperactivity Disorder (ADHD), and dyslexia. In these latter cases, some genetic influence is suspected as these conditions can run in families but the genetic basis is not fully understood. Finally, disorders can be caused by atypical environments, either biochemical (e.g., mothers taking drugs during pregnancy) or psychological (e.g., cases of deprivation or abuse). Notably, some developmental disorders can exhibit very uneven cognitive profiles. For example, there may be particular problems in language but less so in nonverbal areas (e.g., SLI). Some abilities can appear relatively stronger against a background of low IQ (e.g., face recognition in Williams syndrome). How should we explain these uneven profiles?
Where uneven cognitive profiles are observed in typical adults who have experienced brain damage, the usual recourse is to infer that certain parts of the adult cognitive structure have sustained damage. Some researchers have attempted to apply this explanatory framework to developmental disorders, inferring that isolated cognitive components have failed to develop, while the rest of the cognitive system has developed typically. Examples include a Theory of Mind module in autism (Baron-Cohen Reference Baron-Cohen1999; Baron-Cohen et al. Reference Baron-Cohen, Tager-Flusberg and Cohen1993) and a syntax module in SLI (Van der Lely Reference Van der Lely1997). Where the disorder has a genetic basis, there has been a further temptation to view uneven cognitive profiles as evidence for direct links between genes and particular cognitive mechanisms.
Explaining developmental deficits with reference to the typical adult cognitive system is, however, problematic. The adult structure is not prespecified but is itself a product of development. Yet strong analogies with adult brain damage produce accounts of developmental deficits with no role for development at all. In contrast empirical evidence supports the role of development in producing atypical cognitive profiles. When Paterson et al. (Reference Paterson, Brown, Gsödl, Johnson and Karmiloff-Smith1999) explored the language and number abilities of toddlers with Down syndrome and Williams syndrome, they found a different relative pattern to that observed in adults with these disorders. The profile in early childhood was not a miniature version of the adult profile.
The influence of genetic variation and genetic mutation on brain development is not yet fully understood. However, current data suggest that genetic effects are typically graded and diffuse, and have not been found to co-occur with the regions of the cortex associated with specialised higher cognitive functions in typical adults. For example, the British KE family were initially identified as having a specific speech and language deficit caused by mutation to a single gene (FOXP2). However, subsequent research revealed that there were widespread structural and functional brain differences in family members possessing the mutation, while cognitive deficits extended outside the domain of language to negatively affect, for example, performance on nonverbal, rapid associative learning tasks (Watkins et al. Reference Watkins, Dronkers and Vargha-Khadem2002a; Watkins et al. Reference Watkins, Vargha-Khadem, Ashburner, Passingham, Connelly, Friston, Frackowiak, Mishkin and Gadian2002b). In a comparison of a number of genetic syndromes, Kaufmann and Moser (Reference Kaufmann and Moser2000) confirmed that diffuse effects on brain development are the norm.
The neuroconstructivist approach places the developmental process at the heart of explanations of developmental disorders (Karmiloff-Smith Reference Karmiloff-Smith1998a). Empirically, the framework encourages researchers to focus on trajectories of development rather than static snapshots. Theoretically, disorders are viewed as cases of atypically constrained trajectories. A disordered system is still adaptive, yet it may not possess the neurocomputational constraints that are appropriate to acquire a domain. In some circumstances, apparently typical behaviors may be generated by atypical underlying processes (see, e.g., Deruelle et al. Reference Deruelle, Mancini, Livet, Casse-Perrot and de Schonen1999; Karmiloff-Smith et al. Reference Karmiloff-Smith, Thomas, Annaz, Humphreys, Ewing, Grice, Brace, Van Duuren, Pike and Campbell2004, for work on face recognition in Williams syndrome). In other cases, the atypical constraints may produce better than typical performance in a domain, such as in some aspects of perception in autism. In Waddington's (Reference Waddington1957) metaphor, the epigenetic landscape has changed.
Several of the core ideas of neuroconstructivism are emphasized by the study of atypical development. For example, in some cases interactive specialization of cortical areas appears atypical. Adults with Williams syndrome exhibit face recognition skills in the normal range, but examination of ERPs reveal reduced evidence of specialization and localization of neural activity (e.g., Grice et al. Reference Grice, Spratling, Karmiloff-Smith, Halit, Csibra, de Haan and Johnson2001). Neuroimaging data have suggested differences in the constraints of chronotypy, in terms of the changes in connectivity (and associated plasticity) over time in disorders such as autism and Down syndrome (e.g., Becker et al. Reference Becker, Armstrong and Chan1986; Chugani et al. Reference Chugani, Muzik, Behen, Rothermel, Janissee, Lee and Chugani1999).
Differences in input encoding have been proposed to have cascading effects on the context in which other cognitive abilities are acquired (e.g., in autism, SLI, and dyslexia). Alterations in the level of abstraction achieved in forming internal representations, or in the dimensions of similarity that those representations encode, can play a material role in the ability of other brain systems to employ this information to drive other processes. It is possible that in autism, SLI, and dyslexia, for example, the consequence of atypical similarity structure in the input representations results in a processing deficit much higher up in a hierarchy of representational systems. Differences in embodiment may also impact on the trajectory of development. For example, Sieratzki and Woll (Reference Sieratzki, Woll, Greenhill, Hughes, Littlefield and Walsh1998) proposed that in children with spinal muscular atrophy, a disorder that reduces early mobility, language development might be accelerated as a compensatory way for the young child to control their environment. Lastly, an atypical child co-specifies an atypical social environment, for example, in the expectations and reactions of parents and peers, which has also been observed to influence these children's development.
Of course, when we place an emphasis on development as a trajectory, and atypical development as an atypically constrained trajectory, it becomes increasingly important to specify what is different about the constraints and mechanisms of change. Here computational modeling has offered exciting avenues for progress in the study of disorders (e.g., disorders of infant gaze perception: Triesch et al. Reference Triesch, Teuscher, Deák and Carlson2006; disorders of language: Thomas & Karmiloff-Smith, Reference Thomas and Karmiloff-Smith2003).
3.7. Dyslexia
Reading is a relatively recent human invention, going back only a few thousand years. It is highly unlikely that evolution has produced domain-specific constraints on the cognitive systems involved (McCandliss et al. Reference McCandliss, Cohen and Dehaene2003). The existence of a specialised reading system in a brain must therefore represent an adaptation of more general functions to reflect the specific environmental demands of cultures that encourage expertise in this area.
Neuroimaging suggests that reading recruits up to a dozen distinct brain areas (Dehaene Reference Dehaene2003). One particular area, the visual word form area, shows comparably high levels of activity for words and pseudowords (seemingly plausible nonwords made up of standard letters), but not for illegal letter symbols, suggesting an area that processes visual stimuli that look like words, prior to establishing whether they have a meaning (Dehaene et al. Reference Dehaene, Le Clec', Poline, Le Bihan and Cohen2002; Posner et al. Reference Posner, Petersen, Fox and Raichle1988). The location of this area is relatively consistent across individuals and languages (and thus scripts). Because it couldn't have been selected by evolution, this area must be one that happens to have appropriate computational properties for processing words; that is, fine foveal discrimination and invariant recognition of letter- and word-sized stimuli (McCandliss et al. Reference McCandliss, Cohen and Dehaene2003).
The emergence of reading requires a mapping to be established between the linguistic phonological discriminations of the preliterate child and the letters or letter clusters he or she must learn: That is, the child must learn the relation between graphemes (new) and phonemes (old). Some languages, such as English and French, have inconsistent mappings between graphemes and phonemes (e.g., the letter ‘i’ sounds different in the English words bit and bite). Compared to languages with consistent mappings (e.g., Italian and Spanish), inconsistent mappings can delay proficient grapheme-phoneme decoding by up to two years (Goswami Reference Goswami2002; Reference Goswami and Csepe2003).
Reading disabilities in English affect 5 to 17 percent of school-aged children (Shaywitz & Shaywitz Reference Shaywitz, Shaywitz and Swaiman1994). Two main subtypes of developmental dyslexia have been proposed (Castles & Coltheart, Reference Castles and Coltheart1993; Manis et al. Reference Manis, Seidenberg, Doi, McBride-Chang and Petersen1996). Phonological developmental dyslexia involves difficulties reading novel or pseudowords, whereas surface developmental dyslexia describes a difficulty in reading irregular words for which the pronunciation cannot be predicted from the sounds of the individual letters (words such as aisle or yacht).
Twin studies have suggested a significant genetic contribution to developmental dyslexia (Pennington Reference Pennington and Tager-Flusberg1999; Plomin & Dale Reference Plomin, Dale, Bishop and Leonard2000; Plomin & Rutter Reference Plomin and Rutter1998). However, a direct mapping of gene to cognitive function is highly unlikely. Therefore, one might expect to observe more widespread effects than dyslexia alone if there is a genetic aetiology. Although there is no consensus and substantial variability in the literature, especially for surface dyslexia, various concurrent cognitive deficits have been observed in individuals with dyslexia, suggesting a more general sensorimotor syndrome (Stein & Walsh Reference Stein and Walsh1997).
Most computational models of typical and atypical reading development assume that the domain problem constitutes learning to map between the representational codes for written words, spoken words, and word meanings (e.g., Harm & Seidenberg Reference Harm and Seidenberg2004; Plaut et al. Reference Plaut, McClelland, Seidenberg and Patterson1996; Seidenberg & McClelland Reference Seidenberg and McClelland1989). Surface dyslexia has been simulated by altering the initial computational constraints so that the system's ability to learn the mapping between orthography and phonology is reduced. (Sometimes this involves impairing a putative route to pronunciation via word meaning.) Phonological dyslexia has been simulated in two majors ways. The first method is to degrade the properties of the phonological representations (e.g., Harm & Seidenberg Reference Harm and Seidenberg2004). The second method degrades the ability of the system to learn the functional linking orthography and phonology. It is notable that, in this account, similar manipulations can produce symptoms of either surface or phonological dyslexia; many people with dyslexia also show symptoms of both types (Manis et al. Reference Manis, Seidenberg, Doi, McBride-Chang and Petersen1996).
Developmental dyslexia serves to illustrate the principles of neuroconstructivism in the following ways. Reading is a specialisation of a more general system, reflecting the context of a particular environment. In typical development, reading involves dynamic interactions between multiple functions with suitable computational properties. Partial representations interact during development, as highlighted by the restructuring of phonology when the mapping to graphemes is learned. In developmental dyslexia, the somewhat heterogeneous clusters of difficulties reflect the different ways crucial mappings between phonology, orthography, and semantics can be disrupted, as illustrated by computational work. This is consistent with the suggestion of a genetic aetiology, which would be unlikely to selectively disrupt a function that evolution cannot have selected in the first place. Rather, genetic anomalies are expected to show more general, diffuse effects with differential rather than specific consequences in particular domains.
4. Conclusions
Our framework has many implications for developmental theory. One major implication is that our proposal of multilevel isomorphism is a radical rejection of Marr (Reference Marr1982). Cognition cannot be studied independently of the brain and body. Another important implication is the central role of developmental trajectories in the interpretation of adult cognition. There is no teleology involved in development; mature, normative cognition is an outcome of development, not a pre-specified target (Thomas & Karmiloff-Smith Reference Thomas and Karmiloff-Smith2003).
We have also argued that brain regions do not utilize complete representations. In support of this view, we discussed, first, how a particular input signal is typically processed separately along distinct dimensions (e.g., shape, color, motion in object perception), and second, that functional brain systems are interrelated with other functional systems, and are located and within a body and an environment. All these contexts provide varying levels and sources of information such that only fragments of information need to be represented. An implication is that cognition will be compositional and systematic (e.g., Fodor Reference Fodor1975; Fodor & Pylyshyn Reference Fodor and Pylyshyn1988) only if the context permits it.
Progressive specialization, and notions such as emergent modularity (e.g., Karmiloff-Smith Reference Karmiloff-Smith1998a) imply that, as a result of development, the cognitive architecture will exhibit a progressive lack of flexibility to the novel. This can be observed when emergent specialized systems have well-delineated functions (Johnson & Munakata Reference Johnson and Munakata2005). These specialized systems should not be construed as mere imprinting from environmental pressures and regularities. The child, from birth (e.g., Robertson et al. Reference Robertson, Guckenheimer, Masnick and Bacher2004), is an active contributor to his or her development. Our emphasis on context-dependence may be taken as implying that it is impossible to make general claims about cognition. This is not the case. Instead, we argue that the key to understanding contextualised function is to identify those contexts that are central to the function of interest, while ignoring those contexts that may have a peripheral rather than central role in determining the function of interest.
A recurrent theme in our book is the need for causal theories regarding what makes complex behaviors emerge. These theories need to explain behaviors on multiple time scales. They must explain how and why behaviors unfold as we observe them in real time, as well as how they unfold in developmental time. To do this, we need more than just a very detailed description of the behaviors that can be observed at any point. Certainly, such descriptions are essential for the advancement of causal theories of development, but they are unsatisfactory to the extent that they are unable to explain or predict new behaviors. The clearest example of this is with regards to explaining the behavior of children with developmental disorders. Unless one has a mechanistic theory of what is causing behaviors to unfold, and a causal theory of what is atypical in such children's processing, it is impossible to explain or predict why one set of atypically developing children may show a delay at one behavior and excel at another, while a second set of atypically developing children will excel at the former behavior but have a developmental delay in the latter behavior.
In the companion volume, Neuroconstructivism, volume2: Perspectives and Prospects (Mareschal et al. Reference Mareschal, Sirois, Westermann and Johnson2007b), we invited nine research labs with objectives broadly consistent with the neuroconstructivist approach to present their computational modeling work. The questions the models are built to investigate differ both in the level of description and in time scale over which the relevant behaviors operate. Some models focus on relatively rapid adaptation occurring (perhaps) at the cellular level of description, whereas other models focus on relatively slow adaptation occurring at the cognitive level.
We asked all contributors to the companion volume to emphasize the following aspects of their contributions when describing their work:
What functional brain constraints operate on the process of representation development?
What embodiment or situatedness constraints operate on the process of representation development?
Ultimately, computational models are tools to help us reflect on questions of process and mechanisms. Therefore, we also asked the contributing authors to answer the following questions:
How does the model embody these constraints?
What concrete predictions does the model make?
In Neurocontructivism, volume 1: How the brain constructs cognition, we set out to investigate how the representations that underlie cognition emerge in the brain during development. We argued that the emergence of such representations is the outcome of a constructivist process involving constraints that operate at all levels from the cellular environment to the social environment. To truly understand how these representations emerge, it is necessary to locate our theories at the point where the constraints of brain, body, and environment come together.
ACKNOWLEDGMENTS
The writing of this paper was supported by EC grants 516542 (NEST) and 029088 (NEST), EPSRC Grant EP/D062225/1, ESRC grant RES-061-23-0129, MRC grants G9715587 and G0300188, and British Academy grant SG-40400.