Introduction
Commercial use of NSP enzymes in poultry diets started in the late 1980's and early 1990's due to their ability to correct the wet litter and variable apparent metabolisable energy (AME) problem associated with the use of high levels of barley or wheat. Ever since, hundreds of studies have been published exploring the anti-nutritional properties of viscous NSP in certain cereal grains and alleviation of these negative effects by supplementation with suitable endo-acting enzymes. The viscosity argument was so widespread and convincing that the application of NSP enzymes became the norm in situations where appreciable amounts of barley, rye, or wheat were available to the feed industry. This practice continued despite the observations that many wheat varieties during the following years did not pose a serious viscosity challenge, hence a response to supplemental endo-xylanase could not be explained solely in terms of ‘correcting’ the viscosity problem. In fact, this had been noted long ago when comparing three distinct xylanase enzymes in wheat-based diets, some of which reduced viscosity and some which did not, but they all improved performance (Choct et al., Reference CHOCT, KOCHER, WATERS, PETTERSSON and ROSS2004). They suggested the enzyme response could not be related to the viscosity reduction alone and there must be alternative mechanisms that had not been sufficiently explored (Choct et al., Reference CHOCT, KOCHER, WATERS, PETTERSSON and ROSS2004). This opened up a new era of academic and commercial research targeting the exploration of the use of NSP enzymes in non-viscous grains, especially corn. Today, according to a recent global survey, the penetration rate of NSP enzymes in poultry diets has been reported to exceed 70%, suggesting a general acceptance of the feed industry for these enzymes regardless of cereal type.
A variety of product choices are available to the feed industry. These range from mono-component single enzymes to cocktails of more than one activity to so-called ‘complex’ enzymes displaying, in addition to the main activity, several non-targeted (i.e. quality controlled or assured) activities within one product. Broadly speaking, the selection of a product would likely reflect the understanding of the potential role and proposed mode of action of the NSP enzyme in question. Various mechanisms have been suggested to explain the effect of NSP enzymes that include removal of the nutrient encapsulating effect of plant cell-walls, provision of biologically active oligomers with a potential prebiotic role and modulation of the gut micro-flora in addition to viscosity reduction. It is not the intention to describe these mechanisms in detail in this paper, but those interested are referred to the published reviews on this subject matter (Bedford and Morgan, Reference BEDFORD and MORGAN1996; Aftab, Reference AFTAB2012; Courtin, Reference COURTIN2014; Masey O'Neill et al., Reference MASEY O'NEILL, SMITH and BEDFORD2014).
This review revolves around the question of selecting an NSP enzyme, data supporting some of the common views held in the industry today, and how these views significantly influence the process of selecting an NSP enzyme for commercial in-feed application will be discussed.
Consideration of the amount of substrate
A common opinion is to relate the amount, or relative abundance, of the substrate offered by a given dietary raw material as the criterion for selection of an enzyme solution. Although this may make sense in most enzyme-substrate scenarios, there are at least two good reasons to exclude this approach in the case of NSP enzymes: 1) the substrate is not susceptible to the enzyme under the conditions of the animal's gut, or 2) the product/s of the substrate hydrolysis fail to prove, directly or indirectly, beneficial to the host animal. A simple example of the former would be a diet containing high levels of palm kernel meal. A large concentration of mannan, contributing about 40% of the dry weight of palm kernel meal (Back Knudsen, 1997) would suggest mannanase as the enzyme of choice until it is realised that palm-mannan is refractory to the majority of supplemental mannanases (Mok et al., Reference MOK, LEE and KIM2013), hence the total quantity of substrate is meaningless from an enzyme application standpoint. A more typical example of an inert substrate is cellulose that is present in most diets, but the idea of achieving a meaningful hydrolysis of cellulose by means of supplemental cellulase is far from reality in the monogastric gut.
Another example where the quantity of substrate seems to make it an appealing target but where the results are not consistent includes galactosides and pectin. Regardless of the fact that galactosides and pectin constitute about 7 and 20% of the dry weight of soybean meal respectively (Choct et al., Reference CHOCT, DERSJANT-LI, MCLEISH and PEISKER2010), the application of the enzymes resulted in little or no success in improving the technical performance of broilers (Waldroup et al., Reference WALDROUP, FRITTS, KEEN and YAN2005; Reference WALDROUP, KEEN, YAN and ZHANG2006; Tahir et al., Reference TAHIR, SALEH, OHTSUKA and HAYASHI2006; Vieira et al., Reference VIEIRA, OTT, BERRES, OLMOS, CONEGLIAN and FREITAS2006; Ao et al., Reference AO, CANTOR, PESCATORE, FORD, PIERCE and DAWSON2009). This is despite the fact that, in the case of the galactosides, the enzyme failed to deliver a growth response despite significant in-situ (Slominski et al., Reference SLOMINSKI, MENG, CAMPBELL, GUENTER and JONES2006) or in-vitro (Graham et al., Reference GRAHAM, KERLEY, FIRMAN and ALLEE2002) hydrolysis of the substrate.
On the other hand, substrates which appear to be relatively minor constituents of the raw material, may in fact yield far greater benefits if broken down by the relevant enzyme. For example, Cowieson et al. (2010) reported a significant improvement in nutrient and energy digestibility and feed efficiency of broilers in response to supplementation of xylanase or glucanase to a corn-soy based diet. In view of the relative abundance of the substrate, the response to glucanase appears difficult to explain and would likely suggest an involvement of a mechanism independent of the relative quantity of the substrate. The provision of biologically active oligomers could offer at least one plausible explanation to these responses in view of the findings that only a trivial amount of the ‘correct’ oligosaccharide could drive a significant growth response (Courtin, Reference COURTIN2014; Bedford - unpublished).
Consideration of the number of substrates
One of the common approaches is to relate the ‘complexity’ of diet - complexity in this context refers to the presence of a range of different NSP substrates resulting from using alternative feedstuffs in diet formulation - as the basis for selecting an enzyme solution (Meng and Slominski, Reference MENG and SLOMINSKI2005; Cozannet et al., Reference COZANNET, KIDD, NETO and GERAERT2017). A recent Dutch study attempted to look into the effect of supplementation of mono- and multi-component enzymes to simple (wheat-soy) versus complex (wheat-soy, peas, sunflower meal, and canola meal) diets for broilers. The results of the study revealed some interesting observations - a complex enzyme (having several enzyme activities) showed a significant response in the ‘simple’ but not in the ‘complex’ diet (Ten Doeschate et al., Reference TEN DOESCHATE, MASEY O'NEILL and VAN DE BELT2015). On the other hand, one of the mono-component enzymes delivered a significant response in both diet-types while another two single-component enzymes only showed a response in the complex but not in the simple diet. These responses clearly show that ‘tailoring enzyme activities to their substrates to affect a performance outcome’ is a flawed approach. It is not clear whether the NSP in the diet is actually a substrate for the ‘selected’ enzyme under the conditions of the intestinal tract, whether NSP is indeed an anti-nutrient and whether the products of enzyme hydrolysis (if indeed it is active) are beneficial or detrimental.
Meng and Slominski (Reference MENG and SLOMINSKI2005) noted an improved total tract digestibility of NSP as a result of supplemental complex enzymes in both corn-soybean meal or corn-canola meal-based diets (i.e. a ‘good-fit’ to the diets, arguably). However, the improved NSP digestibility coincided with improved ileal digestibility of protein in the corn-soy diet while depressing the protein digestibility in corn-canola based diet which was reflected in an improved growth rate and efficiency in corn-soy diet with no effect in corn-canola meal based diets. Another study, exploring the effect of NSP enzymes and different vegetable protein meals revealed a significant reduction in the feed intake and body weight gain when a complex enzyme was used on a diet containing cottonseed meal, while no effect was observed when the major protein meal was soybean, canola, or sunflower (Aftab, Reference AFTAB2009). One possible inference of these observations is that some enzyme activities in a complex enzyme might end up producing compounds with possible undesirable effects. An indiscriminate hydrolysis of dietary NSP could prove detrimental and certain NSP fractions would be better left to pass ‘intact’ through the gut (e.g. Vahjen et al., Reference VAHJEN, BUSCH and SIMON2005).
On the other hand, a complex diet involves the use of alternative feed ingredients which are often characterised by lower and/or variable nutritional quality e.g. rapeseed meal or corn distillers dry grains and solubles (DDGS). In this context, an improved magnitude or consistency of an enzyme response may well be explained in terms of an increased undigested fraction (Cowieson and Bedford, Reference COWIESON and BEDFORD2009; Bao et al., Reference BAO, ROMERO and COWIESON2013) rather than the ‘complexity’ of the substrate per se. Hence it seems likely that introduction of poorly digestible alternative ingredient to a test diet may increase the rate of success of an enzyme supplementation (Sultan et al., Reference SULTAN, GAN, LI, ZHANG and BRYDEN2011; Romero et al., Reference ROMERO, SAND, INDRAKUMAR, PLUMSTEAD, DALSGAARD and RAVINDRAN2014; Olukosi et al., Reference OLUKOSI, BEESON, ENGLYST and ROMERO2015) but for reasons that do not necessarily relate to the complexity of their NSP.
In-vitro substrate hydrolysis
In vitro substrate hydrolysis studies are generally based on work presenting visual evidence of cell-wall degradation (Masey O'Neill et al., Reference MASEY O'NEILL, SMITH and BEDFORD2014; Ravn et al., Reference RAVN, MARTENS, PETTERSSON and PEDERSEN2016) or increased release of reducing sugars after incubating feed samples in an enzyme solution (Meng et al., Reference MENG, SLOMINSKI, NYACHOTI, CAMPBELL and GUENTER2005). Microscopic evidence often shows erupted or thinner plant cell walls in treatment groups compared with intact cell walls in the untreated controls. However, often these assays are characterised by using a very high dose of enzyme, choosing the ‘ideal’ assay conditions for the enzyme in question, prolonged incubation and ensuring the absence of the interacting factors that would normally be present in the gut and may confound the in-situ substrate hydrolysis. Given such divergence from the in vivo versus in vitro dosage and assay conditions these data end up contributing little to the debate.
In-vivo substrate hydrolysis
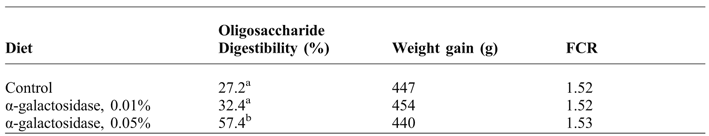
Often in vivo digestibility of the substrate is used as an indicator of the justification for use of an enzyme candidate. Although interesting from a viewpoint of academic research, it is worth asking if the extent of substrate hydrolysis has a direct correlation with technical performance of the target animal. For example, a significant hydrolysis of substrate which does not lead to improved animal performance has minimal value in terms of in-feed applications (Table 1; Slominski et al., Reference SLOMINSKI, MENG, CAMPBELL, GUENTER and JONES2006).
In-vivo substrate hydrolysis and the growth performance.

a-b P<0.05; Slominski et al. (Reference SLOMINSKI, MENG, CAMPBELL, GUENTER and JONES2006)
Targeting extensive NSP-hydrolysis would make sense if the hydrolytic end products is available as a direct source of useful energy to the animal, but this proposition is questionable on two fronts. First, the possibility of achieving complete enough substrate hydrolysis under the constraints of an animal's gut is remote at best; and second, the possible pre- and post-absorptive fate of the constituent monosaccharides of the most relevant NSP fractions of practical diets would make the idea of an extensive substrate hydrolysis undesirable (discussed further below).
Fate of mono-sugars
Despite the limitations in the practicality of achieving an extensive substrate fibre hydrolysis in the monogastric gut, there is evidence suggesting the end products of complete hydrolysis of some NSP fractions are poorly metabolised by poultry. There may even be circumstances where an increased release of some of these monosaccharides proves detrimental to the growth rate and efficiency of the animal (Schutte, 1990; Regassa et al., Reference REGASSA, KIARIE, SANDS, WALSH, KIM and NYACHOTI2016). For example, studies involving supplementation of xylose in chicken (Schutte, Reference SCHUTTE1990) or galactose in rat (Cori, Reference CORI1925) diets have shown about 50% of the absorbed sugars were excreted via the urine, suggesting monogastric animals have a poor ability to metabolise these sugars. Furthermore, feeding xylose and arabinose was associated with an increase proliferation of microflora in the small intestine and incidence of wet droppings in poultry perhaps as a result of the slower rate of absorption of these sugars compared with glucose (Schutte, Reference SCHUTTE1990). These observations would suggest that NSP enzymes are not classical ‘digestive’ enzymes and hence their efficacy may not be related of the extent of substrate hydrolysis achieved.
Prebiotic sugar generation
More recently it has been proposed that the generation of prebiotic oligosaccharides by NSP enzymes is largely responsible for the growth promoting effects observed, particularly in low viscosity diets (Courtin et al., Reference COURTIN, BROEKAERT, SWENNEN, LESCROART, ONAGBESAN, BUYES, DECUYPERE, VAN DE WIELE, MARZORATI, VERSTRAETE, HUYGHEBAERT and DELECOUR2008; Lee et al., Reference LEE, APAJALAHTI, VIENOLA, GONZALEZ-ORTIZ, FONTES and BEDFORD2017). This is thought to improve animal performance through direction of the microbiome to a structure more favourable to optimal performance and reduced likelihood of pathogenic challenge. It is interesting that Rosen (Reference ROSEN2010) predicted that NSP enzymes would function more effectively in diets which did not contain an antibiotic - an empirical observation which tends to support such a hypothesis. If this hypothesis is correct then the goal of NSP enzyme inclusion in a diet is not hydrolysis per se, but generation of specific oligosaccharides. Such a hypothesis further challenges the need for multiple endo-acting enzymes to generate multiple oligosaccharide types if one type (e.g. arabino-xylo-oligosaccharides, AXOS; Courtin et al., Reference COURTIN, BROEKAERT, SWENNEN, LESCROART, ONAGBESAN, BUYES, DECUYPERE, VAN DE WIELE, MARZORATI, VERSTRAETE, HUYGHEBAERT and DELECOUR2008) can deliver the response on their own. More importantly, it suggests that the goal should be a hydrolytic action which is limited in extent such that oligosaccharides are generated but not further degraded to shorter and less effective disaccharides or monosaccharides which are no longer prebiotic. Dose and type of enzymes would be important as much as the absence of any exo-acting enzymes which may depolymerise oligosaccharides thereby rendering them inactive at best and an anti-nutrient at worst if reduced to a monosaccharide. The future direction of NSP enzyme discovery would be better placed targeting the products released by the enzyme rather than the extent of hydrolysis achieved should this hypothesis dominate, and, if so the future may see NSP enzyme supplemented with or supplanted by exogenous oligosaccharides.
Do additional enzyme activities strengthen a xylanase response?
Several commercial enzyme product choices are available on the market. Most, if not all of these have xylanase as a key activity, which asks the question as to whether this is the ‘sole essential activity’ or whether the presence of additional activities is necessary in order to render the product effective. The term ‘sole essential activity’ has been used here to clarify that most fermentation processes produce several ‘side’ activities, the presence of which do not always warrant their ‘effectiveness’ as a feed enzyme. This simple demarcation helps separate multi-enzyme products developed from a single fermentation to those cocktails tailored by combining separate activities each obtained from specific fermentation process. In this section, we shall discuss only the latter category (the ‘customised cocktails’) since there is no way the biological relevance of the side-activities in the former can be established scientifically.
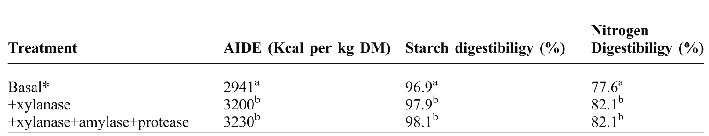
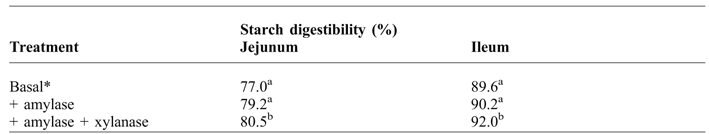
Some xylanase products have been supplemented with protease and or amylase activities, based on these additional activities helping to digest the starch and protein ‘released’ by the opening-up of the plant cell wall by xylanase. The key assumption for this proposal that the endogenous supply of protease and amylase is insufficient in the chicken gut under normal circumstances and needs augmentation from an exogenous source, is however, open to question (Moran, Reference MORAN1982; Reference MORAN1985; Noy and Sklan, Reference NOY and SKLAN1995; Svihus, Reference SVIHUS2014). Although some references point to the usefulness of amylase for young broiler chicks (Gracia et al., Reference GRACIA, ARANIBER, LAZARO, MEDEL and MATEOS2003), the effects these early-age benefits have on final body weight or feed efficiency is not clear. In fact, evidence to support the benefit of additional ‘endogenous’ enzyme activities is insufficient to the best of our knowledge and is confounded by the fact that very few studies have been published with a design giving the reader an opportunity to separate the response of each constituent activity in a cocktail. Tables 2 and 3 summarise results of two recent studies which meet such a criterion and demonstrated that the digestibility of N and starch or ileal digestible energy was improved by xylanase, while an addition of amylase or amylase combined with protease had no effect thereby challenging the assumption that there was an insufficient supply of endogenous amylase or protease.
The value of the additional enzyme activities.

*Corn 63-68%, soybean meal 32-27%, meat & bone meal 1.7-2.3%; Amerah et al. (Reference AMERAH, ROMERO, AWATI and RAVINDRAN2017)
a,b P<0.05
DM=dry matter
The value of the additional enzyme activities.

*Corn 54%, soybean meal 36%; Stefanello et al. (Reference STEFANELLO, VIEIRA, SANTIAGO, KINDLEIN, SORBARA and COWIESON2015)
a,b P<0.05
The question of additional NSP enzyme activities in improving the response to a solitary xylanase response was addressed by Cowieson et al. (2010). The data from their study highlighted the lack of an additive response when glucanase was combined with xylanases in a typical corn-soy diet.
Correct response indicator?
In addition to performance, research often includes a wide range of response criteria in order to look into the potential mechanistic and interacting effects. These alternative response criteria are valuable only when a significant correlation with growth performance measures is established. There have been circumstances where a potentially positive response in terms of one criterion actually resulted in a depression, rather than an improvement, of another important index. For example, an increased faecal score of bifidobacteria and lactobacilli resulting from feeding a pre-biotic was in fact coupled with a significant reduction in the ileal and total tract digestibility of dry matter, organic matter, and N (Smiricky-Tjardes et al., Reference SMIRICKY-TJARDES, GRIESHOP, FLICKINGER, BAUER and FAHEY2003). Another example, the co-occurrence of an improved villus height and crypt depth with depressed growth performance has been reported in recent pig work from Michigan State University (Moeser, Reference MOESER2016). Indeed, an increased intestinal volume could be regarded as an advantage in terms of an increased absorptive surface as well as a disadvantage in view of more nutrients needed for their maintenance, so the eventual ‘usefulness’ of an increased villus height and crypt depth, or any other index for that matter, would remain unproven unless it also translates into an improved gain or efficiency of feed utilisation.
Similarly, improvements in the nutrient digestibility may also need to be interpreted with caution since these do not take into account the ‘intake’ effect and are simply a point-in-time measurement which may or may not reflect a long-term effect on the growth rate and efficiency of an animal. Of significance to NSP enzymes could be the situation where the hydrolytic end products could not be utilised efficiently, or at all, by the host animal. For example, failure of a large improvement in the true metabolisable energy of soybean meal with supplemental alpha-galactosidase to translate into improved growth rate and efficiency of broilers (Graham et al., Reference GRAHAM, KERLEY, FIRMAN and ALLEE2002). It is likely that some of the key benefits associated with feeding of an NSP enzyme e.g. altered caecal fermentation, modulation of the gut flora, digesta passage rate and retention time within each segment of the digestive tract will not be captured by ‘classical’ digestibility assays. Alternatively, there is the question as to whether achieving the highest degree of pre-caecal nutrient digestibility is always a desirable target. For example, the negative effect of reduced pre-caecal starch digestibility by introducing certain resistance starch (RS) into a diet may partly be ameliorated by the potential prebiotic effect of RS in the hindgut (Giuberti et al., Reference GIUBERTI, GALL, MOSCHINI and MASOERO2015). Indeed, the classical digestibility assays fail to take into account these small, but long-term, and hence significant, effects on growth performance.
Consistency of an enzyme response
The consistency of beneficial responses to an enzyme is one of the key considerations from a commercial point of view, which can be confounded by the fact that negative or not significant trials do not usually get published, and hence a review of published literature suggests an erroneously high rate of ‘success’ (Aftab, Reference AFTAB2012). Consistent benefits depend upon the magnitude of any challenge under which the birds are grown, e.g. the concentration of viscous NSP in the diet, basal diet digestibility, or degree of gut insult. For example, the most suitable model to study the effect of an endo-xylanase would be to use a rye-based diet fed under ‘dirty’ rearing conditions. In this particular case, one would expect a marked and highly consistent response, the predominant part of which could be attributed to the removal of tangible viscosity and pathogenic challenge due to poor hygiene. If a relatively ‘milder’ challenge e.g. reduced viscosity challenge as a result of using barley or wheat instead of rye as the sole dietary cereal, and rearing under moderate challenge which simulates commercial rearing, then the magnitude, as well consistency of the response would likely decline. The enzyme response in this case would possibly involve a combination of the viscosity-reduction and modulation of the gut flora. In dietary models posing a negligible viscosity challenge i.e. corn- or rice-based diets coupled with cleaner, stress-free rearing conditions (such as University/pen trials research) would result in a further muting of the enzyme response both in terms of magnitude and consistency. This would translate into less FCR improvement and occurrence; the most likely explanatory factor being the hind-gut fermentation and modulation of the microbial balance in the gut.
It appears that modulation of the gut flora is central to the response to the supplemental NSP enzymes in non-viscous diets and explains a large part of the puzzle surrounding ‘consistency’ of the enzyme responses.
Conclusions
The aim of this review was to discuss the data supporting some of the common views held in the industry today, and how these views significantly influence the process of selecting an NSP enzyme for commercial in-feed application. The relative abundance of the substrate or the number of substrates presented by a given diet and the extent of in vitro or in vivo substrate hydrolysis may not serve the sole criteria for selecting an NSP enzyme. The idea of having additional non-NSP or NSP activities to ‘strengthen’ a xylanase response, as well as the notion ‘complex diet needs a complex enzyme’ appear to lack sufficient scientific backing. Measures based on alternative responses e.g. gut morphology, nutrient or energy digestibility, gut-flora and its metabolites or fermentation profiles, are useful in developing a wider understanding of the phenomenon but require careful interpretation as the stand-alone criteria of usefulness of an NSP enzyme. Performance data is always the ultimate judge of the efficacy of a feed enzyme.