Ecological studies on galling insect species diversity in the Neotropics show that galling species richness depends on biotic factors related to floristic diversity (Araújo et al. Reference ARAÚJO, SCARELI-SANTOS, GUILHERME and CUEVAS-REYES2013, Cuevas-Reyes et al. Reference CUEVAS-REYES, QUESADA, HANSON, DIRZO and OYAMA2004, Fernandes & Price Reference FERNANDES and PRICE1988, Mendonça Reference MENDONÇA2007), such as plant structural complexity, plant density, plant ontogenetic stage, plant composition and plant species richness (Araújo et al. Reference ARAÚJO, SANTOS and GOMES-KLEIN2012, Reference ARAÚJO, SCARELI-SANTOS, GUILHERME and CUEVAS-REYES2013; Cuevas-Reyes et al. Reference CUEVAS-REYES, QUESADA, HANSON, DIRZO and OYAMA2004, Fernandes & Price Reference FERNANDES and PRICE1988, Oyama et al. Reference OYAMA, PÉREZ-PÉREZ, CUEVAS-REYES and LUNA-REYES2003). However, there is confusion in the literature concerning the hierarchical importance of these factors at both local and regional scales (McGeoch & Price Reference McGEOCH and PRICE2005, Oyama et al. Reference OYAMA, PÉREZ-PÉREZ, CUEVAS-REYES and LUNA-REYES2003).
A relative consensus in the studies of galling insects indicates that plant species richness is one of the most important factors explaining the variation in galling richness at the regional scale (Araújo et al. Reference ARAÚJO, SCARELI-SANTOS, GUILHERME and CUEVAS-REYES2013, Gonçalves-Alvim & Fernandes Reference GONÇALVES-ALVIM and FERNANDES2001, Oyama et al. Reference OYAMA, PÉREZ-PÉREZ, CUEVAS-REYES and LUNA-REYES2003). It is not difficult to understand that the changes in plant richness between different localities influence galling richness, as observed in Neotropical savannas (Araújo et al. Reference ARAÚJO, SCARELI-SANTOS, GUILHERME and CUEVAS-REYES2013, Gonçalves-Alvim & Fernandes Reference GONÇALVES-ALVIM and FERNANDES2001). In contrast, the occurrence of a particular plant species or genus at the local level can influence the diversity patterns that increase galling species richness, because these plants might host a greater number of galling species, sometimes being called super-hosts (Araújo et al. Reference ARAÚJO, SANTOS and GOMES-KLEIN2012, Reference ARAÚJO, SCARELI-SANTOS, GUILHERME and CUEVAS-REYES2013; Mendonça Reference MENDONÇA2007, Veldtman & McGeoch Reference VELDTMAN and McGEOCH2003). The reasons why a genus or species is a super-host is still not clear. However, emergence of these plant taxa may be due to developmental synchrony and the sympatric occurrence of its species (Araújo et al. Reference ARAÚJO, SCARELI-SANTOS, GUILHERME and CUEVAS-REYES2013). The synchrony between sympatric hosts favours the phenomenon of oviposition error that is considered an important mechanism in galling-insect speciation (Mendonça Reference MENDONÇA2007). Therefore, the presence of super-host taxa can increase the local galling richness, even if plant richness is low, because they represent keystone resources to galling insects (Araújo et al. Reference ARAÚJO, SCARELI-SANTOS, GUILHERME and CUEVAS-REYES2013). A similar effect can be expected for plant abundance on the local richness of galling, although at the regional scale, the presence of super-host taxa does not appear to be a determining factor (Araújo et al. Reference ARAÚJO, SCARELI-SANTOS, GUILHERME and CUEVAS-REYES2013).
Despite recent advances in the study of the effects of plant species richness and the presence of super-host taxa on galling insect diversity (Araújo et al. Reference ARAÚJO, SANTOS and GOMES-KLEIN2012, Reference ARAÚJO, SCARELI-SANTOS, GUILHERME and CUEVAS-REYES2013; Mendonça Reference MENDONÇA2007), the relative importance of these factors at both the local and regional levels remains unclear in the ecological literature. Therefore, in this study, we determined the effects of plant species richness, plant abundance and super-host presence on the local and regional galling richness in Neotropical savannas. In particular, we tested the following hypotheses: (1) galling insect richness is influenced by plant species richness only at regional scale, and (2) at local scale, factors related to plant abundance and super-host abundance are the most important to galling richness.
Galling insect richness and host plant species diversity were sampled in 15 areas of Neotropical savanna in the States of Distrito Federal, Goiás, Minas Gerais and Tocantins, Brazil (Araújo et al. Reference ARAÚJO, SCARELI-SANTOS, GUILHERME and CUEVAS-REYES2013). The sampled areas were distributed in a large latitudinal range (11–19°S) with the areas closest located 10 km apart. In each area, we randomly established 10 plots of 10 × 10 m (at least 50 m apart), in which we sampled all woody plants with a girth greater than 15 cm at ground level. We used this criterion because these plants were previously identified to vegetation monitoring, besides being easier to identify and quantify. Each plant sampled was catalogued in the field, and we recorded all galls on leaves, stems and flowers. We used the gall morphotypes as surrogates for galling insect species based on: (1) host plant species; and (2) morphological characteristics of the galls (e.g. organ appearance, size, colour and pubescence) (Araújo et al. Reference ARAÚJO, SCARELI-SANTOS, GUILHERME and CUEVAS-REYES2013, Cuevas-Reyes et al. Reference CUEVAS-REYES, QUESADA, HANSON, DIRZO and OYAMA2004). This approach is based on the relative consensus in the literature about the host-specificity and morphology-fidelity of insect galls (Cuevas-Reyes et al. Reference CUEVAS-REYES, QUESADA, HANSON, DIRZO and OYAMA2004). We used the genus Qualea (Vochysiaceae), represented by three species in this study, as a super-host taxon because recent studies in Neotropical savannas show that species of this genus have three times more galling diversity than the other plant species (Araújo et al. Reference ARAÚJO, SANTOS and GOMES-KLEIN2012, Reference ARAÚJO, SCARELI-SANTOS, GUILHERME and CUEVAS-REYES2013).
We used multiple regression models and AIC selection criteria to test the relationship between the explanatory variables plant richness, plant abundance and abundance of Qualea and the galling insect richness. At the regional level, we used each area as a sampling unit (N = 15) and at the local level, we performed particular analyses using the plots within each sampled area (N = 10). For these analyses we used the residuals of relationship between plant richness and plant abundance, to evaluate the effect of plant species richness that is independent of the total number of plants in each area or plot. To meet normality requirements, we applied the logarithmic transformation to plant abundance both at regional and local scales. In order to control the spatial dependence of our data, we performed a spatial autocorrelation analysis of all variables, but we found no significant spatial autocorrelation.
We sampled 131 species and 43 families of plant, 48% of which (64 species and 31 families) hosted 112 galling insect species. The greatest number of gall morphotypes recorded occurred in leaves (83.9%), compared with stems (13.4%) and other organs (2.7%). Vochysiaceae, Fabaceae and Malpighiaceae were the families that hosted the greatest galling richness, with 19, 13 and 12 gall morphospecies, respectively. The species of Qualea had mean ± SD of 6 ± 2.6 galling morphotypes, while the other species had mean of 1.5 ± 0.9. The overall mean was 1.8 ± 1.4.
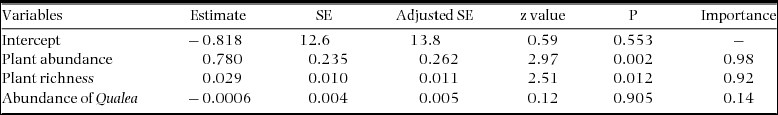
At the regional level, the only model selected that explained the galling insect richness included plant species richness and plant abundance (df = 3, AICc 97.07, ∆AICc < 0.01). At this scale, the explanatory variables plant richness and plant abundance had high and similar importance (0.92 and 0.98, respectively; Table 1). On the other hand, the abundance of Qualea had little importance (0.14).
Statistical values and importance of explanatory variables in the multiple regression model explaining galling insect richness at the regional level in Neotropical savanna in Brazil. The importance indicates the relative explanatory power of each variable.

We found that the patterns of galling species richness were different at the local level. At this level, plant abundance and/or abundance of Qualea were present in the best models selected to explain the galling richness in 80% of the sampled areas. These variables were the most important in 80% and 14% of the areas, respectively. In none of the studied areas did plant richness have high importance or was it selected as a component of the best models.
Our results showed that the relative importance of plant-related factors to galling species richness is different at regional and local levels. We corroborate the idea that plant species richness is an important predictor of galling richness at the regional level (Araújo et al. Reference ARAÚJO, SCARELI-SANTOS, GUILHERME and CUEVAS-REYES2013, Oyama et al. Reference OYAMA, PÉREZ-PÉREZ, CUEVAS-REYES and LUNA-REYES2003), but not at local level. Differences in plant species pools between local communities and regional flora might explain the observed results. Although local communities sometimes have a pool of species, which represent a significant portion of the regional species pool (Lewinsohn & Roslin Reference LEWINSOHN and ROSLIN2008), most often the local pool is much smaller than the regional one (Gramling Reference GRAMLING2006). Thus, the limited species pool at the local level causes the plant species richness to vary little between different plots. Furthermore, there is evidence that different plots of a local community might have a greater substitution of plant species, even though the number of species in these plots remains constant (Bakker et al. Reference BAKKER, OLFF, WILLEMS and ZOBEL1996). Alternatively, at the regional level, the species pool may be much higher, which produces great variation in the number of species across different localities (Felfili et al. Reference FELFILI, SILVA-JÚNIOR, SEVILHA, FAGG, WALTER, NOGUEIRA and REZENDE2004). Therefore, at the regional level, the larger species pool and the great variation in the plant richness between localities, can be determinants of the galling species richness, whereas other factors can be important at the local level.
We found evidence that at the local level the plant abundance is the main factor that explains the galling insect richness. Our study represents a major advance compared with previous studies (Araújo et al. Reference ARAÚJO, SCARELI-SANTOS, GUILHERME and CUEVAS-REYES2013, Oyama et al. Reference OYAMA, PÉREZ-PÉREZ, CUEVAS-REYES and LUNA-REYES2003) because it is the first to directly analyse the relationships between host-plant abundance per species and the number of galling species in different areas of the Brazilian savannas. One possible mechanism that explains our results is that conspecific trees are hosts of similar galling insect faunas, and that plants at high density have a greater probability of being found by herbivores than isolated plants or plants at low abundance (Hyatt et al. Reference HYATT, ROSENBERG, HOWARD, BOLE, FANG, ANASTASIA, BROWN, GRELLA, HINMAN, KURDZIEL and GUREVITCH2003).
We also observed that the abundance of Qualea at the local level was positively related to galling species richness in some communities. This genus was sampled in 13 of the 15 study areas, confirming the observations that Qualea species are the plants found with higher frequency in areas of Neotropical savanna (Ratter et al. Reference RATTER, BRIDGEWATER and RIBEIRO2003). A great diversity of galling insects has been documented to be associated with species of Qualea (Gonçalves-Alvim & Fernandes Reference GONÇALVES-ALVIM and FERNANDES2001) and some evidence shows that the occurrence of this host genus significantly influences local galling richness (Araújo et al. Reference ARAÚJO, SCARELI-SANTOS, GUILHERME and CUEVAS-REYES2013).
Our findings confirm recent results that plant richness is the main predictor of galling species richness at the regional level (Araújo et al. Reference ARAÚJO, SCARELI-SANTOS, GUILHERME and CUEVAS-REYES2013), whereas the composition and structure of the vegetation play a secondary role. To the best of our knowledge, our study represents a major advance to previous studies because it is the first to directly identify the importance of local and regional plant traits as determinants of the galling insect richness. Most studies that have evaluated gall-plant interactions on different scales only addressed this issue in an indirect or circumstantial way (Araújo et al. Reference ARAÚJO, SCARELI-SANTOS, GUILHERME and CUEVAS-REYES2013, Oyama et al. Reference OYAMA, PÉREZ-PÉREZ, CUEVAS-REYES and LUNA-REYES2003). We found that local factors, such as the abundance and distribution of super-host taxa and the number of host plants, are important factors to explain the variation in local galling insect species richness. However, we suggest that further study or meta-analyses of data in the literature might increasingly clarify the local and regional patterns of galling insect distribution.
ACKNOWLEDGEMENTS
We thank Ian Turner, Leonardo Bergamini and an anonymous reviewer for constructive suggestions, CAPES for the grant to W.S. Araújo, and CNPq for a productivity grant to F.A.G. Guilherme.