Introduction
The fruit fly Anastrepha ludens Loew (Diptera: Tephritidae) is a major pest of mango (Mangifera indica L.) and Citrus spp. fruits in Mexico and Central America (Hernández-Ortiz, Reference Hernández-Ortiz1992, Reference Hernández-Ortiz, Aluja and Liedo1993; Hernández-Ortiz & Aluja, Reference Hernández-Ortiz and Aluja1993; Aluja, Reference Aluja1994). To control it, a National Programme has been implemented since 1992 in Mexico, using an area-wide pest control strategy, where the sterile insect technique (SIT) is a key element (Orozco-Dávila et al., Reference Orozco-Dávila, Domínguez, Reyes, Villaseñor, Gutiérrez and Barnes2004; Gutiérrez, Reference Gutiérrez, Montoya, Toledo and Hernández2010). The application of the SIT requires mass-production, sterilization and release of males of the target species. Its success depends critically upon the ability of released sterile males to mate with wild females under natural field conditions. This requires that sterile males survive long enough in the field, find and join leks, and court and mate wild females (McInnis et al., Reference McInnis, Shelly and Komatsu2002). However, the effects of laboratory colonization and mass-rearing conditions during many generations could adversely affect field survival and performance. These adverse effects have been found in the courtship and mating behaviour of mass-reared males (Harris et al., Reference Harris, Wood, Bailey, Mangel, Carey and Plant1986, Reference Harris, Wood and Bailey1988; Whittier et al., Reference Whittier, Nam, Shelly and Kaneshiro1994; McInnis et al., Reference McInnis, Lance and Jackson1996; Cayol, Reference Cayol, Aluja and Norrbom2000; Eberhard, Reference Eberhard, Aluja and Norrbom2000; Lux et al., Reference Lux, Munyiri, Vilardi, Liedo, Economopoulos, Hasson, Quilici, Gaggl, Cayol and Rendon2002; Rull et al., Reference Rull, Brunel and Mendez2005); the synchronization of their sexual activity (Miyatake, Reference Miyatake1998, Reference Miyatake2011; Shelly et al., Reference Shelly, Rendón, Hernández, Salgado, McInnis, Villalobos and Liedo2003); and their ability to avoid predators (Hendrichs et al., Reference Hendrichs, Wornoayporn, Katsoyanos and Hendrichs2007; Dor et al., Reference Dor, Valle-Mora, Rodríguez-Rodríguez and Liedo2014).
To overcome these limitations, several authors (McInnis et al., Reference McInnis, Shelly and Komatsu2002; Rull et al., Reference Rull, Brunel and Mendez2005) proposed alternative colonization strategies: (1) to replace the mass-rearing adapted strain with a new one starting from wild founders (replacement); (2) infusion of wild male behaviourally desirable traits into mass-rearing adapted females by crossing wild males with mass-reared females (hybrid); and (3) using selected males for their sexual competitiveness as strain founders (selected).
In Ceratitis capitata (Wied.), Shelly (Reference Shelly2001) found that crossing wild males with mass-reared adapted females resulted in F1 hybrid males that were as competitive as wild ones, but the F10 hybrid males showed reduced competitiveness, similar to the long-time mass-reared adapted males. McInnis et al. (Reference McInnis, Shelly and Komatsu2002) found in the same species a strong positive response to selection and hybridization by mass-reared males that successfully mated with wild females. The selection and hybridization process was repeated in alternate generations in four cycles and the positive effect lasted at least for 30 generations. Since the independent effect of selection and hybridization was not measured, authors proposed to evaluate the two processes separately, over multiple generations. Rull & Barreda-Landa (Reference Rull and Barreda-Landa2007) found that first-generation hybrids of A. ludens wild males and mass-reared females were more sexual competitive than mass-reared males. The effect of selection on mating performance was evaluated by Bosa et al. (Reference Bosa, Cruz, Zepeda-Cisneros, Valle-Mora, Guillén-Navarro and Liedo2016) on only one generation, and Quintero-Fong et al. (Reference Quintero-Fong, Toledo, Ruiz, Rendón, Orozco-Dávila, Cruz and Liedo2016) and Sánchez-Rosario et al. (Reference Sánchez-Rosario, Pérez-Staples, Toledo, Valle-Mora and Liedo2017) on four generations, showing that selection improved sexual performances of offspring. Tejeda et al. (Reference Tejeda, Arredondo, Liedo, Pérez-Staples, Ramos-Morales and Díaz-Fleischer2016) evaluated the effect of selection on resistance to desiccation, showing that A. ludens is able to adapt rapidly to desiccation stress, reducing its impact on reproduction capability.
Until recently, the effects of colonization and colony management methods have focused on the mating competitiveness of mass-reared males, but not on their ability to survive to predators. This trait can drastically jeopardize survival probabilities of mass-reared sterile males, in particular when sterile males have to survive several days in the field before reaching full sexual maturity. Predation might be the most important mortality factor on sexually active males (Burk, Reference Burk1982) and it could be one of the selection factors that resulted in lek mating systems (Bradbury, Reference Bradbury, Alexander and Tinkle1981). Hendrichs (Reference Hendrichs1986) found that A. suspensa (Loew) courting males were more predated than females and males on the periphery of leks compared with those in the centre. Hendrichs & Hendrichs (Reference Hendrichs and Hendrichs1998) reported predation by wasps on pheromone-calling C. capitata males.
González-López et al., (Reference González-López, Rao, Díaz-Fleischer, Orozco-Dávila and Pérez-Staples2016) found 18 families of spiders in Mexican citrus orchards where the Mexican fruit fly was common. The most abundant spider families were Salticidae, Anyphaenidae and Thomisidae. In semi-field conditions, sterile males of the unisexual strain of A. ludens (Tapachula-7) (Zepeda-Cisneros et al., Reference Zepeda–Cisneros, Meza Hernández, Palacios, Martínez, de León Crisóstomo and Flores-García2014) showed a lower survival than fertile wild males in the presence of the orb-web spider Leucauge venusta (Araneae: Tetragnathidae) (González-López et al., Reference González-López, Rao, Díaz-Fleischer, Orozco-Dávila and Pérez-Staples2016).
In this study, we focused on another potential natural predator that is common in Mexican fruit fly habitats: the orb-weaver and diurnal spider Argiope argentata Fabricius 1775 (Araneae: Araneidae). The spider is widely distributed in Central and South America (Levi, Reference Levi1968). Females are up to 35 mm in length and males reach <20 mm (Robinson, Reference Robinson1969). Their cephalothorax is silver coloured on the dorsal side; the dorsal abdomen is decorated with brown, black and orange coloured point at the posterior extremity. In the field, the orb-web is almost symmetrical, inclined at 5°–20° from the vertical axis, and its size varies according to location and time (≈20 cm diameter for adults). The typical position of the mature spider on its web is hanging on the underside of the hub, in a characteristic cruciform attitude. The four pairs of legs are in line with the stabilimenta, which are formed of bands of zigzag silk and are in the form of a diagonal perpendicular cross (Lubin, Reference Lubin1975). Craig et al. (Reference Craig, Wolf, Davis, Hauber and Maas2001) reported polymorphism in the web decoration. This spider species regularly preys on Diptera (Robinson, Reference Robinson1969; Robinson & Robinson, Reference Robinson and Robinson1970). When a spider detects an entangled fly in the web, it generally attacks wrapping the fly in silk and biting it with its jaws. Then, the spider cuts the prey package from the web and carries it in its jaws towards the hub, where it is wrapped again and consumed (Robinson & Olazarri, Reference Robinson and Olazarri1971).
Our aim in this study was to assess the ability of A. ludens males originating from different colony establishment approaches to survive predation by A. argentata under laboratory standard conditions. We compared the predator survival ability of males coming from replacement, hybrid and selected colonies, plus mass-reared and wild males as controls. Our hypothesis was that males obtained from a selection process (selected) and males with wild inheritance (replacement and hybrid) were better at avoiding predators than mass-reared males and as good as wild males.
Material and methods
Biological material
Anastrepha ludens: Wild individuals were collected as larvae from infested grapefruits and sour oranges gathered from small orchards or backyards around Tapachula city, Chiapas, Mexico. Fruits were brought into the laboratory, where larvae completed their development and were manually extracted and counted 8 days later. They were placed in containers with vermiculite to allow pupation. After 14 days, pupae were placed in open Petri dishes inside 30 × 30 × 30 cm3 glass cages for adult emergence. The Petri dishes with the empty pupal cases and non-emerged pupae were removed from the cages after 24 h, so the age of all the flies in each cage was the same (within 24 h). The adults were fed ad libitum with a standard 3:1 sugar: enzymatically hydrolysed yeast solid diet (Hagen & Finney, Reference Hagen and Finney1950). Water was provided in plastic vials (10 cm long and 2.7 cm diameter) plugged with wet cotton. To avoid unexpected effects due to high density, a maximum of 400 adults were kept per cage. Laboratory environmental conditions were 26 ± 2°C temperature, 80 ± 10% relative humidity, and 12:12 h light–dark cycle. Wild flies were used as positive control.
A second control (mass-reared flies) and three experimental strains (replacement, hybrid and selected) were managed under the same laboratory conditions. Mass-reared parental flies were obtained from the Moscafrut mass-rearing facility (SAGARPA-IICA) located in Metapa, Chiapas, Mexico. This facility produces around 120 million sterile A. ludens flies per week as part of the actions of the National Fruit Fly Programme (Domínguez et al., Reference Domínguez, Artiaga, Solís, Hernández, Montoya, Toledo and Hernández2010; Orozco-Dávila et al., Reference Orozco-Dávila, Quintero, Hernández, Solís, Artiaga, Hernández, Ortega and Montoya2017). The original colony was derived from a hybrid between a 10-year-old colony from Texas and wild flies from six different Mexican states (Orozco-Dávila et al., Reference Orozco-Dávila, Hernández, Meza and Domínguez2007). At the moment of this study, the Moscafrut colony was 16 years old. Males were separated from females. Adults were maintained in cages as described above.
The replacement strain was obtained from the initial cross of 1000 sexually mature wild males and 1000 sexually mature wild females into five 30 × 30 × 30 cm3 glass cages (200 flies of each sex per cage) under laboratory conditions. We facilitated oviposition, providing ‘simulated fruits’ with green fucelleron (gel) (Burtonite 44, Tic Gums; Inc. Madison, USA) spheres wrapped with parafilm® (Hernández et al., Reference Hernández, Toledo, Artiaga-López and Flores2009). Eggs were collected from these egging devices and placed on a standard diet until larvae finalized their development. Then they were treated as described above for wild and mass-reared pupae. The hybrid strain was obtained from the initial cross of 1000 wild males and 1000 mass-reared females (from the Moscafrut mass-rearing facility) in a 70 × 18 × 45 cm3 rearing cage with a vertical fabric board covered with fucelleron as oviposition device (Hernández et al., Reference Hernández, Toledo, Artiaga-López and Flores2009). Rearing conditions and procedures were similar to those used at the Moscafrut facility (Domínguez et al., Reference Domínguez, Artiaga, Solís, Hernández, Montoya, Toledo and Hernández2010; Orozco-Dávila et al., Reference Orozco-Dávila, Quintero, Hernández, Solís, Artiaga, Hernández, Ortega and Montoya2017).
The selected strain was derived from mass-reared parental flies and was obtained from two initial selection filters that were based on survival and sexual competitiveness of mass-reared males under field cage conditions. In four mesh field cages (3 m diameter and 2.2 m high), a total of 800 mass-reared newly emerged males (200 per cage) were released and left there during 4 days. Predators as small ants and small spiders that were able to enter through the mesh were not removed from the cages. Inside each cage, six to eight small mango trees were placed to provide a resting area, and 20 droplets of food solution were provided on the surface of 20 leaves (one drop per leaf in a 1:1 water: food ratio; food was a 3:1 sugar: hydrolysed yeast mixture). At the 4th day, there were eight surviving males that were collected and brought back to the laboratory where they were maintained with ad libitum access to the standard laboratory diet and water in glass cages until they reached sexual maturity (14 days old). Then, they were brought once again into the field cages together with eight wild sexually mature females from 16:00 to 20:00 h. The three males that were able to mate were recaptured (99.625% selection pressure) and placed in glass cages with three virgin sexually mature mass-reared females per male to found the selected strain. The offspring eggs of these selected males were reared under standard conditions, as described above, and tested.
The selection, hybridization and replacement colonies were made only once, in the parental generation, but their offspring were reared during six consecutive generations. Tests were made with individuals from these six generations of each strain. Since we found no effect of generation, the data were pooled and generations were considered as replicates.
Argiope argentata: Mature females of about 35 mm of body length were captured in the low herbages and shrubs at the edges of a grapefruit plantation at the Rosario Izapa experimental station of the ‘Instituto Nacional de Investigación Forestales, Agricolas y Pecuarias’ (14°58′28″ N and 92°9′16″ W). Their webs were identified by the conspicuous cross stabilimenta. Female spiders were collected in vials and brought to the laboratory, where they were maintained under the same conditions as the fruit flies. Each individual was held in a 30 × 30 × 30 cm3 glass cage in which a 21 cm diameter vertical metallic ring was installed in the centre as a frame for web construction. This ring was maintained vertically with two plastic screw caps in which the ring was inserted. Spiders were able to weave their orb-web in <24 h, using the ring and cage walls as supports. Water was supplied in impregnated cotton wool on a Petri dish and was sprayed every 2 or 3 days on cage walls and the web. Five living mass-reared fruit flies were introduced every 5 days in each cage to feed the spiders. This amount of flies was sufficient to maintain spiders well fed. Remains of dead fruit flies were removed every 5 days to avoid the arrival of carnivorous ants. Preliminary experiments showed that spiders needed at least 15 days to adapt themselves to the standard conditions.
Preliminary experiment
Five flies were introduced in each cage with one spider. The number of surviving flies was recorded at 0, 1, 2, 3, 4, 6, 8, 22, 26, 28, 32, 46, 48, 55, 70 and 78 h. The spiders were food deprived for 5 days prior the test. Ten replicates were done.
Survival of wild and mass-reared A. ludens males
We tested the survival of wild and mass-reared males of similar maturity level, exposing them simultaneously to one spider. Flies were marked on the thorax with a different colour of acrylic paint to allow differentiation (Aluja et al., Reference Aluja, Jacome and Macias-Ordoñez2001). Wild males were 4–37 days old and mass-reared males were 3–30 days old. In each 30 × 30 × 30 cm3 cage, four individuals of each strain were placed together with one spider for 6 h in 39 trials. Preliminary experiments showed that out of a total of five fruit flies, 2.20 ± 0.33 were eaten per spider in this time period (N = 10, spiders were previously food deprived for 5 days).
After the 6 h period, the number of surviving fruit flies was recorded and they were removed from the cages. We considered that spiders killed all the remaining flies in the cage: entangled or silk packed flies in the spider's web, the flies that were reduced to the form of small light brown pellets on the cage floor (remains of not consumed tissues of the fly such as exoskeleton and wings) and the immobile flies on the floor with the characteristic crossed dead limbs’ position. Each predator was used more than once during trials, but they were food deprived for 3 or 5 days between trials. Webs used for the experiment were constructed with foundation threads, a spiral zone, an attachment zone, and a hub (see Robinson & Olazarri, Reference Robinson and Olazarri1971). When spiders died, or when they did not show normal behaviours, such as when they did not weave adequate orb-web, they were replaced.
Survival of A. ludens males from five experimental strains
We tested simultaneously the survival of marked A. ludens males of the five strains (wild, mass-reared, replacement, hybrid and selected) in the presence of one spider. Wild males were 7–47 days old, mass-reared males: 10–54 days old, replacement males: 5–45 days old, hybrid males: 10–46 days old and selected males were 10–46 days old. In total, we ran 228 fruit fly–spider confrontations. In each encounter, three males of each A. ludens strain were exposed to the spider, for a total of 15 fruit flies that were simultaneously exposed per each spider and confrontation. At the end of each confrontation, the surviving and healthy fruit flies (which were not captured by the predator) were collected and recorded.
Data analysis
Preliminary experiment
We calculated the mean number ± standard error of eaten fruit flies by the ten spiders for each record time. A descriptive variation analysis was done, calculating the line slope during the first 6 h of the confrontation and until all the flies were consumed (Δ eaten fruit fly number/Δ hours of confrontation). This slope represented the predation rate.
Survival of wild and mass-reared A. ludens males
The effect of the strain (wild or mass-reared males) was analysed with a generalized mixed linear model with the R statistical program (R Core Team, 2013). A likelihood ratio test (χ2) was used to evaluate the effect of the strain on the survival distribution (binomial). Since spiders were used more than once, we considered them as a random variable in the model.
Survival of A. ludens males from five experimental strains
The survival of males of the five A. ludens strains (wild, mass-reared, replacement, hybrid and selected) was analysed with a generalized mixed linear model with the R statistical program. A likelihood ratio test (χ2) was used to evaluate the effect of the strain on the survival distribution (binomial). Spiders were used as random variables. Contrast comparisons were made with an ad hoc Tukey test, using an adjust alpha of 0.01.
Results
Preliminary experiment
Figure 1 shows the predation rate from the preliminary experiment. During the first 6 h, the number of preys consumed increased rapidly. The mean number of flies consumed per spider was 2.20 ± 0.33 fruit flies. Afterward, the predation rate levels off. All five flies were consumed within the 78 h period. Considering that 40% of the flies were consumed in the first 6 h, we determined that a 6 h period was enough to assess the survival ability of the flies.
Mean of eaten mass-reared A. ludens flies (± standard error) exposed to one A. argentata spider during 78 h.

Survival of wild and mass-reared A. ludens males
Survival to predation by A. argentata depended on fruit fly strain. The mass-reared fruit fly males were less likely to survive (0.29 ± 0.005) after an encounter with the spider than wild fruit flies (0.55 ± 0.064) (table 1, fig. 2).
Estimated mean survival probability (± standard error) of A. ludens males of five strains (wild and mass-reared) exposed to one A. argentata spider.

Likelihood ratio test of fruit fly males survival as a function of fruit fly strains (W, wild; MR, mass-reared; H, hybrid; R, replacement; S, selected) against Argiope argentata spiders.

Survival of A. ludens males from five experimental strains
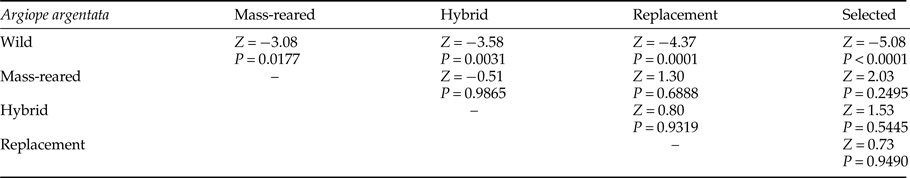
Fruit fly strain affected the probability of being predated by A. argentata (table 1). Survival abilities of wild males were significantly higher than that of the males of the other strains (table 2, fig. 3).
Estimated mean survival probability (± standard error) of A. ludens males of five strains (wild, mass-reared, hybrid, replacement and selected) exposed to one A. argentata spider.

Contrast comparisons with ad hoc Tukey test of the estimated mean survival probabilities of males of the five strains against Argiope argentata spiders. α = 0.01.

Discussion
A. argentata spiders were easy to find in the field, they are common and easy to identify through the conspicuous cross-shaped stabilimenta of its web. They were also easy to maintain under standard laboratory conditions. The detection of the flies captured by the spider was also easy, since they were entangled, silk packed or their remains fell down on the cage floor, forming a small ball of organic matter (diameter 2–3 mm). For these reasons, this spider species is a good candidate to assess the ability to avoid spider predation in quality control evaluations of mass-reared fruit flies.
When presented to spiders, mass-reared fruit fly males had a lower survival than wild males. The greater survival of wild flies could be attributed to their ability or strength to escape from the web. Another reason could be their greater activity level. Rao et al. (Reference Rao, Aguilar-Argüello, Montoya and Díaz-Fleischer2013) showed that non-irradiated mass-reared A. ludens were less likely to perform a supination to deter the jumping spider Phidippus audax (Hentz) and to avoid it than wild A. ludens. We confirmed that mass-rearing conditions affect the ability of males to avoid predation, as was reported for non-irradiated and irradiated A. ludens males from the bisexual strain and irradiated Tap-7 males (González-López et al., Reference González-López, Rao, Díaz-Fleischer, Orozco-Dávila and Pérez-Staples2016), and C. capitata (Hendrichs et al., Reference Hendrichs, Wornoayporn, Katsoyanos and Hendrichs2007). These results are also in line with the reduction of mating competitiveness of mass-reared males vs. wild males (McInnis et al., Reference McInnis, Lance and Jackson1996; Rull et al., Reference Rull, Brunel and Mendez2005), meaning that the colonization process affects the field survival and sexual performance of sterile males. The absence of predators at the mass-rearing facility and laboratory conditions may explain this decreased capacity to survive natural enemies (O'Steen et al., Reference O'Steen, Cullum and Bennett2002; Schmidt et al., Reference Schmidt, Krivan and Ovadia2004). Wild males showed high survival ability, suggesting a constant selection pressure in nature that selects individuals permanently alert and apt to evade predation risks.
Results from comparison of the five strains showed different patterns for each individual spider, however, overall the different colony establishment approaches did not improve survival ability, since there were no significant differences in the performance of males exposed to the spider, and always lower than that of wild males.
As the replacement colony had recent wild individuals, we expected that replacement males would show similar survival ability as wild males. Nevertheless, results showed that the adaptation bottle-neck from wild males to mass-rearing conditions was drastic and might be related to a decrease in the evasion ability of the flies (Pinson et al., Reference Pinson, Tejada, Toledo, Enkerlin, Celedenio-Hurtado, Valle-Mora, Pérez and Liedo2006 for A. serpentina; Liedo et al., Reference Liedo, Salgado, Oropeza and Toledo2007 for C. capitata; Hernández et al., Reference Hernández, Toledo, Artiaga-López and Flores2009 for A. obliqua). Results obtained for the hybrid males, which have mass-reared mothers, showed that they also had lower survival than wild males in the presence of spiders.
Selected males did not show the expected good survival abilities. This strain had the lowest survival values, suggesting that the selection process used did not favour their survival ability. These results differ from the mating competitiveness of males from the same selected population, they were better sexual competitors than mass-reared males (Sánchez-Rosario, Reference Sánchez-Rosario2013). Other studies showed the advantage of selecting males to improve their sexual competitiveness (Bosa et al., Reference Bosa, Cruz, Zepeda-Cisneros, Valle-Mora, Guillén-Navarro and Liedo2016; Quintero-Fong et al., Reference Quintero-Fong, Toledo, Ruiz, Rendón, Orozco-Dávila, Cruz and Liedo2016; Sánchez-Rosario et al., Reference Sánchez-Rosario, Pérez-Staples, Toledo, Valle-Mora and Liedo2017). In our study, the capacity of selected males to evade one orb-weaving spider in a confined space (0.33 m3) was poor. One possible explanation is that males were not selected for their ability to avoid predation. They were selected to survive under limited food and water availability and under the environmental conditions of a field cage. Perhaps, predation risk was low, spiders and ants were small and other natural predators, such as larger orb-weaving spiders or actively hunting wasps (Hendrichs & Hendrichs, Reference Hendrichs and Hendrichs1998) and dwelling lizards (Dor et al., Reference Dor, Valle-Mora, Rodríguez-Rodríguez and Liedo2014), could not enter the cage due to their large size. Indeed, if we compare the survival of male C. capitata in a citrus orchard vs. inside a field cage within the same orchard, the mortality was much higher for males in the orchard outside the field cage (Hendrichs et al., Reference Hendrichs, Wornoayporn, Katsoyanno and Gaggl1993). Predation pressure may explain these losses in the orchard.
An additional explanation may be that selection took only place for one generation during which some of the few surviving males could have stayed alive due to chance events. Probably selection needs to be applied for a number of generations (McInnis et al., Reference McInnis, Shelly and Komatsu2002), or even continuously as part of a permanent filter system with larger numbers, as it is routinely used to maintain the stability of mother colonies of genetic sexing strains (GSSs) (Fisher & Cáceres, Reference Fisher, Cáceres and Tan2000; Franz, Reference Fisher, Cáceres and Tan2005), so that predator evasion traits are maintained in the genetic makeup of the colony. Furthermore, this selection should preferably take place under semi-natural field cage conditions, and add more predator species involved in the selection process to maintain as much as possible survival traits within a mass-rearing colony flies.
Another issue may be the existence of a trade-off between mating and survival abilities in fruit fly males (Lima & Dill, Reference Lima and Dill1990; Magnhagen, Reference Magnhagen1991; Lima, Reference Lima1998; Lind & Cresswell, Reference Lind and Cresswell2005). A male that evades better a predator and survives may compensate by competing less successfully for mates, or a good mating competitor male may evade or escape predation less successfully. If such trade-off mechanism exists, it will have important repercussions in maintaining important field performance traits of mass-rearing colonies. In the field, mass-reared sterile males will be under predation risk and they will have to compete with wild males for mating with wild females. Therefore, if colonization and colony management strategies are used to maintaining survival and mating performance behaviours in mass-reared sterile males, they should consider applying simultaneously selection pressures to enhance both, survival skills, including the ability to avoid and escape predators, and mating competitiveness.
McInnis et al. (Reference McInnis, Shelly and Komatsu2002) demonstrated that hybrid and selected C. capitata males mated two to three times more than wild males. An interesting avenue to test should be the maintenance of both the survival and mating competitiveness traits of hybrid/selected A. ludens males raised under close to natural conditions over generations. The selection process could include two filters. First, parental flies would be exposed to natural predators such as wasps, orb-weaving spiders or lizards in field cages. Environmental conditions and predator presence will be the selection factors. Second, the surviving males would be selected based on their mating competitiveness. Only the offspring of double selected males and selected females would be allowed to reproduce and enter the mass-rearing colony. Tests of survival, including predator avoidance, and mating abilities should be regularly performed to assess their offspring.
A recent technological advancement in SIT for A. ludens control has been the development of the Tapachula-7 GSS that allows the release of males only (Zepeda-Cisneros et al., Reference Zepeda–Cisneros, Meza Hernández, Palacios, Martínez, de León Crisóstomo and Flores-García2014). Sterile males of this strain are as sexually competitive as the standard bisexual strain (Orozco-Dávila et al., Reference Orozco-Dávila, Meza, Zepeda, Solís and Quintero-Fong2013), but they are less competitive than selected mass-reared males (Bosa et al., Reference Bosa, Cruz, Zepeda-Cisneros, Valle-Mora, Guillén-Navarro and Liedo2016). To improve the GSS, hybridization with wild males will be complicated, since the trait that allows sorting of males and females needs to be maintained (Leftwich et al., Reference Leftwich, Kokidou, Rempoulakis, Gong, Zacharopoulou, Fu, Chapman, Economopoulos, Vontas and Luke2014). Then, colony establishment and maintenance systems based on close to natural conditions and routine selection of the best performing individuals can be an alternative. Effectively, selection based on mating competitiveness in Tapachula-7 GSS A. ludens improved the sexual performance of their offspring (Quintero-Fong et al., Reference Quintero-Fong, Toledo, Ruiz, Rendón, Orozco-Dávila, Cruz and Liedo2016).
Another important factor, not assessed here, to take into account in the future, is the possible effect of irradiation over the performance of sterile flies, since it has been reported that irradiation can affect survival ability (Hendrichs et al., Reference Hendrichs, Wornoayporn, Katsoyanos and Hendrichs2007 for C. capitata), sexual competitiveness (Rull et al., Reference Rull, Brunel and Mendez2005 for A. ludens) and anti-predator behaviour (Rao et al., Reference Rao, Aguilar-Argüello, Montoya and Díaz-Fleischer2013). Also, exposing sterile males to hormonal treatment before release to accelerate sexual maturation (Pereira et al., Reference Pereira, Yuval, Liedo, Teal, Shelly, McInnis and Hendrichs2013), and releasing them closer to sexual maturity, to minimize predation before reproduction (McInnis et al., Reference McInnis, Paranhos and Shelly2013), will be complementary approaches to mitigate the lower predator avoidance and escape abilities of sterile males resulting from mass-rearing conditions.
In conclusion, colonization and mass-rearing conditions have a very strong effect in reducing predator avoidance abilities of A. ludens males. Sterile males that retain behaviours that facilitate the avoidance of predators or escape when attacked by predators will have a greater probability of surviving to reproduce. This needs to be considered when designing colonization and mass-rearing procedures at mass-rearing facilities in order to assure the performance of the resulting sterile males and therefore, the effectiveness and efficiency of the SIT.
Acknowledgements
We are grateful to Reyna E. Bustamente-Girón, Ezequiel De León-Cigarroa, Uriel Gallardo-Ortiz, Lucero. A. Martinez-Moyao, Azucena Oropeza-Cabrera, Rodrigo Rincon-Bermudez, Gustavo Rodas-Bello, Sandra Luz Rodríguez-Alvarez, Susana Rodríguez-Rodríguez, and Mayren Sánchez-Rosario, for technical assistance. Fruit flies were provided by the Moscafrut facility (SENASICA – SAGARPA – IICA). Financial support was provided by the Mexican Consejo Nacional de Ciencia y Tecnología – Fondo Sectorial de Investigación para la Educación (CONACYT, Project 134651). We thank Javier Francisco Valle-Mora for help with statistical analysis. Comments and suggestions from anonymous reviewers contributed to greatly improve the manuscript quality. Spiders were maintained under laboratory conditions in accordance with Mexican official norm NOM-062-ZOO-1999 for the use of experimental animals.