Introduction
Biological invasions are complex processes in which the success of an invasive species depends on introduction to a suitable location followed by successful establishment and dispersion (Lounibos, Reference Lounibos2002). One of the best described examples of animal adaptation to the urban environment is that of the mosquito Aedes aegypti (Linnaeus, 1762), which acts as the principal vector of the dengue, Chikungunya, Yellow Fever and Zika viruses. The A. aegypti mosquito is an invasive species originating from Egypt that spread throughout the Americas, Europe, Asia and Pacific Islands beginning in the 17th century (Brown et al., Reference Brown, Evans, Zheng, Obas, Barrera-Martinez, Egizi, Zhao, Caccone and Powell2014). The most striking behavioral attribute of this mosquito, which can be observed throughout the range of expansion, is its ability to adapt to anthropogenic conditions (Powell & Tabachnick, Reference Powell and Tabachnick2013). Hufbauer et al. (Reference Hufbauer, Facon, Ravigne, Turgeon, Foucaud, Lee, Rey and Estoup2012) postulated that invasive species pre-adaptation led to the development of traits that contribute to increased dispersal of invasive species populations. Human-altered environments directly contribute to this pre-adaptation by enhancing the reproductive success of invasive species in cities compared to more rural environments (Hufbauer et al., Reference Hufbauer, Facon, Ravigne, Turgeon, Foucaud, Lee, Rey and Estoup2012).
In the case of A. aegypti, broad adaptation to the urban environment is probably associated with behavioral traits that allow the species to choose between micro- and macrohabitats. Females of this species prefer to oviposit in man-made containers (e.g., tires, bottles, plastic cups) instead of natural oviposition sites (e.g., bromeliads, tree holes) (Forattini & Brito, Reference Forattini and Brito2003), which is in part associated with a strong preference for human blood (Mcbride et al., Reference McBride, Baier, Omondi, Spitzer, Lutomiah, Sang, Ignell and Vosshall2014); this suggests that human environments and urban conditions selected for those mosquitoes possessing traits that facilitated the colonization of cities. However, one important question regarding the behavioral ecology of synanthropic species such as A. aegypti is how environmental characteristics influence the oviposition behavior of gravid mosquito females. Water-holding containers that can serve as potential oviposition sites are typically spread throughout residences and can be found both indoors and outdoors. In addition to holding water, these microcosms may contain particulate organic matter that can be used as a food source for mosquito larvae (Bentley et al., Reference Bentley, McDaniel, Lee, Stiehl and Yatagai1976).
Mosquito females are able to evaluate potential breeding sites prior to making decisions about egg deposition (Silberbush & Blaustein, Reference Silberbush and Blaustein2008; Silberbush et al., Reference Silberbush, Markman, Lewinsohn, Bar, Cohen and Blaustein2010). High organic matter concentrations in water sources may indicate a profitable site for mosquito females to lay eggs (Bentley & Day, Reference Bentley and Day1989). Thus, it is expected that mosquitoes should prefer to lay eggs in sites with higher organic matter content when available (Ponnusamy et al., Reference Ponnusamy, Wesson, Arellano, Schal and Apperson2010). Laboratory assays have verified this pattern for A. aegypti females (Albeny et al., Reference Albeny-Simões, Murrell, Elliot, Andrade, Lima, Juliano and Vilela2014); however, some studies show that under field conditions, domestic populations of A. aegypti are not able to discriminate among containers with and without organic matter (Leahy et al., Reference Leahy, Vandehey and Booth1978). Indiscriminate oviposition site choice may represent an evolutionary strategy for exotic mosquito species, especially inside human residences where water used for consumption and other daily needs is typically subject to treatment or filtration. This behavior can increase the use of habitats such as water fountains (Silva, Reference Silva2004) and drinking water storage containers (Forattini & Brito, Reference Forattini and Brito2003) by A. aegypti females, thereby increasing the probability of mosquitoes locating appropriate oviposition sites indoors (Powell & Tabachnick, Reference Powell and Tabachnick2013). This has direct implications for the vector potential of this species, as the ability to colonize indoor residential habitats should increase contact rates with humans.
The preference of domestic populations of A. aegypti for human blood compared to other vertebrates (Mcbride et al., Reference McBride, Baier, Omondi, Spitzer, Lutomiah, Sang, Ignell and Vosshall2014) certainly contributed to the successful establishment of this species in urban environments around the world. The strong capability to colonize indoor habitats (Lima-Camara et al., Reference Lima-Camara, Honório and Oliveira2006), combined with the strong preference for human blood (Mcbride et al., Reference McBride, Baier, Omondi, Spitzer, Lutomiah, Sang, Ignell and Vosshall2014) and capability to use water sources for human use suggests that (i) A. aegypti females prefer to lay eggs in containers located inside residences compared with outside; (ii) will show no preference for containers with or without OM content inside of houses; and (iii) will show preference for containers with higher OM outside.
Materials and methods
Study site
We ran oviposition choice assays at residences in the city of Chapecó, Santa Catarina, Brazil (fig. 1). The city is located in the western portion of southern Brazil and is characterized by dense A. aegypti populations during most of the year. We choose residential sampling sites that exhibited similar characteristics such as no mosquito netting on the windows, no AC units, and the presence of a backyard with at least some covered area. We confirmed that the local vector control agency did not employ any physical or chemical control or sampling methods in these areas from two weeks prior through the duration of the experiment, and the inhabitants of the selected homes were informed prior the beginning of the experiment that they should not use any pesticide products (i.e., either for control in the home or skin repellents) during the experimental period.
Location of the city of Chapecó, SC, Brazil and the eight houses where the oviposition containers were installed.

Experimental design
Eight houses were arbitrarily chosen in the city (fig. 1). Each house was considered as an independent experimental unit and received two pairs of oviposition containers placed one meter apart both inside and outside of the home. The oviposition container pairs inside of the house were placed in the main living area. The container pairs outside of the house were placed in the back yard. To assure that the outside oviposition containers was not affected by rainwater, they were placed under covered areas of the yards. If the back yard had no covered area, another house as chosen in the same neighborhood. The oviposition containers were inspected once per week for 9 weeks.
Oviposition containers
The oviposition containers consisted of 1-l capacity, black plastic cups holding 500 ml of water, and the walls of the containers were lined with 5 × 15 cm white seed germination filter paper as an oviposition substrate (Albeny et al., Reference Albeny-Simões, Murrell, Elliot, Andrade, Lima, Juliano and Vilela2014). Oviposition containers were supplied with 500 ml of water plus 7-day-old dried leaf infusion (mixed species, field-collected in the region). The clean water treatment (CWT) received 500 ml of tap water. The turbid water treatment (TWT) received 250 ml of water and 250 ml of leaf infusion. These dilutions generated an organic matter proportion of 0 and 50% for the CWT and TWT, respectively.
Egg sampling
The eggs were sampled weekly by removing the oviposition paper from each oviposition container. A new oviposition filter paper was then placed in the containers and water plus infusion was replaced in the CWT and TWT containers. All of the oviposition containers were rinsed with tap water before refilling with water and leaf infusion for the next experimental week. All sampled eggs were hatched, and larvae were raised to adulthood for identification. Unhatched eggs were not able to be identified.
Analysis
Oviposition activity index
To evaluate the oviposition preferences of females, we used the well-described oviposition activity index (OAI) (Kramer & Mulla, Reference Kramer and Mulla1979). The OAI standardizes the data by converting the numbers of eggs placed in both CWT and TWT containers to proportions, as follows:
 $${\bf OAI}\, = \,({\bf nTWT} - {\bf nCWT})\,/\,({\bf nTWT}\, + \,{\bf nCWT})$$
where nTWT is the number of eggs laid in the TWT and nCWT is the number of eggs laid in the CWT. The OAI varies between −1 to +1, where 0 indicates no preference. Positive values indicate a higher preference for the TWT containers, while negative values indicate a higher preference for the CWT containers.
One-way ANOVA
In addition to the OAI, we analyzed the effects of the independent variables CWT and TWT on the proportion of eggs laid (= response variable). We used generalized linear models, which allowed us to evaluate the error distribution and test for overdispersion, which led us to adjust the data distribution for the quasibinomial family (Crawley, Reference Crawley1993). The analyses were carried out separately for each week for the outdoor oviposition containers. All analyses were carried out using R (R Development Core Team R, 2014).
Two-way ANOVA
A two-way ANOVA was used to analyze the effects of the containers holding TWT and CWT, early season (ES) and late season (LS), and the containers×season interaction (independent variables) on the proportion of A. aegypti eggs laid (response variable). We used Tukey post-hoc test to contrast the mean proportion of A. aegypti eggs laid among the treatments (independent variables).
Repeated measures ANOVA
We perform a repeated-measures ANOVA to evaluate the effects of container location (indoor vs. outdoor) sampling week, and the interaction (independent variables) on the total number of A. aegypti eggs laid (response variable). For this analysis, the response variable (= total number of eggs) was tested for normality using the Shapiro-Wilk test.
Results
General results
We collected a total of 18,465 A. aegypti eggs, of which 15,304 (82.8%) were laid in containers outside of houses and 3161 (17.2%) were laid in containers inside the houses. The CWT and TWT containers received a total of 5565 and 12,900 eggs, respectively (tables 1 and 2).
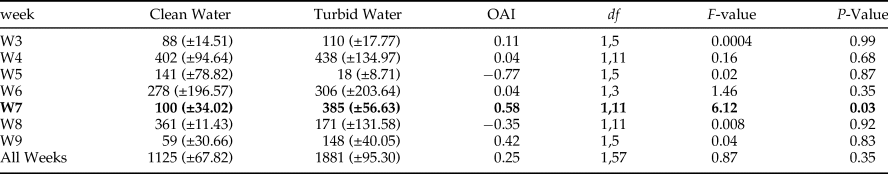
One-way ANOVA showing A. aegypti oviposition preference for outside containers holding clean (CWT) or turbid (TWT) water in each experimental week and all weeks pooled together.

The total number of eggs ± standard deviation are shown for each CWT and TWT. Ovipositional activity index (OAI) values showing the preference for either CWT (negative values) or TWT (positive values), degrees of freedom (df), F and P values are shown in bold. Significant and marginally significant results are shown in bold.
One-way ANOVA showing A. aegypti oviposition preference for inside containers holding clean (CWT) or turbid (TWT) water in each experimental week.

Total number of eggs ± standard deviation are shown for each CWT and TWT. Ovipositional activity index (OAI) values showing the preference for either CWT (negative values) or TWT (positive values), degrees of freedom (df), F and P values are shown in bold.
Inside vs outside containers
We found a significant effect of site location (outside vs. inside) (F 1,201 = 18.77, P < 0.001) and sample week (F 8,192 = 3.54, P = 0.0007) on the total number of eggs laid, but there was no week: site interaction (F 8,184 = 1.05, P = 0.39). The total number of eggs was significantly higher in containers outside than inside houses, especially in the seventh, eighth and ninth sample weeks (fig. 2).
Total numbers of Aedes aegypti eggs laid per week indoors (open circles) and outdoors (closed circles). Error bars represent standard deviation.

Outside container oviposition results
We found no effect of organic matter content on mosquito oviposition choice during the first, third and fourth sample weeks. During the second week, there was a strong oviposition preference for CWT. During the remaining weeks (5 to 9), there was a preference for TWT (table 1, fig.3). Because this strong preference was observed during the last six experimental weeks, we reanalyzed the data using a factorial design pooling together weeks 1- (‘early season’) and weeks 6–9 (‘late season’), considering the potential for the presence/absence of organic matter (TWT/CWT) during the early season vs late season affecting mosquito oviposition choices. There was a significant effect of treatment (F 1,133 = 10.13, P = 0.001), TWT and CWT, and treatment: season interaction (F 1,130 = 11.11, P = 0.001) on the percentage of eggs laid in between seasons. During the early season, the proportion of eggs laid did not differ between TWT and CWT. During the late season, there was a preference for containers with organic matter (fig. 4a).
Oviposition (oviposition activity values) of Aedes aegypti gravid females in clean water and turbid water containers within nine weeks (W1-9) in the outside treatments. All weeks treatment is a result of all of the experimental weeks pooled together. *P < 0.05, ns, nonsignificant.

Proportion of Aedes aegypti eggs laid during the Early season (open circles) and Late season (closed circles) in oviposition container without (No) and With (Yes) organic matter. Left, outside experiment (a) and right, inside experiment (b). Error bars represent standard deviation.

Inside container oviposition results
There was a preference for TWT only during the week seventh. During the remaining periods, no oviposition preferences were observed (fig. 5, table 2). To treat the data consistently, we used the same factorial design described in the previous experiment. None of the variables affected the proportion of eggs laid (fig. 4b). However, there was a significant effect of the treatment: season interaction on the proportion of eggs laid (F 1,64 = 4.74, P = 0.03).
Oviposition (oviposition activity values) of Aedes aegypti gravid females in clean water and turbid water containers over experimental periods inside homes.. The ‘all weeks’ treatment is a result of all of the experimental weeks pooled together. *P < 0.05, ns, nonsignificant.

Discussion
Contrary to our first prediction, A. aegypti eggs were far more numerous in outdoor containers., and there was a strong preference for turbid water compared to clean water in the outdoor containers. This result is strongly supported by the literature, as gravid females are known to have a positive response to chemical cues for bacterial content emanating from oviposition containers (Bentley et al., Reference Bentley, McDaniel, Lee, Stiehl and Yatagai1976; Eitam et al., Reference Eitam, Blaustein and Mangel2002; Albeny et al., Reference Albeny-Simões, Murrell, Elliot, Andrade, Lima, Juliano and Vilela2014). This is because high concentration of organic matter in oviposition water represents a profitable environment for the growth of bacteria (Ponnusamy et al., Reference Ponnusamy, Xu, Nojima, Wesson, Schal and Apperson2008; Ponnusamy et al., Reference Ponnusamy, Wesson, Arellano, Schal and Apperson2010), which serve as a food resource for mosquito larvae (Bentley & Day, Reference Bentley and Day1989). Alternatively, there was no preference for oviposition in CWT or TWT in indoor containers except during the final week of the experimental period. This indicates a strong preference for TWT containers (fig. 5). As this experiment was done in the field under natural conditions, there are a few ways to interpret and discuss the results.
To exert choice, mosquito females must have free access to oviposition containers. In Brazil, residences of most houses do not use mosquito nets and homes generally do not have central air conditioning systems; thus, most people leave the windows and doors opened throughout the day allowing mosquitoes to easily enter homes. However, our results based on egg collection follows a well-known aspect of A. aegypti female biology, which is that females feed indoors because humans live indoors and oviposit outdoors because the majority of the available containers are located outdoors. Previous studies have shown that adult mosquitoes, especially engorged females, are typically found more frequently indoors than outdoors (Lima-Camara et al., Reference Lima-Camara, Honório and Oliveira2006), and this trend seems to be common for A. aegypti populations worldwide (Scott et al., Reference Scott, Morrison, Lorenz, Clark, Strickman, Kittayapong, Zhou and Edman2000). Thus, if the females are already indoors, it is expected that they would search, locate and lay their eggs in indoor containers. This generates an important question in the discussion of mosquito ecology and behavior. For those mosquitoes that choose to lay their eggs in outdoor containers, the selection of containers holding water with low organic matter concentration (i.e., conditions similar to water for daily human use) might not be a priority and that containers with higher organic matter content would be preferred due to availability of resources for offspring development. On the other hand, mosquitoes indoors may utilize available containers irrespective of organic matter concentration simply because there are likely fewer oviposition sites available indoors. . Albeny et al. (Reference Albeny-Simões, Murrell, Elliot, Andrade, Lima, Juliano and Vilela2014), in a series of laboratory experiments, showed that additional input of animal organic matter (conspecific carcasses) produced a highly attractive environment for gravid A. aegypti females. The addition of grass infusion to containers has also been shown to attract ovipositing A. aegypti (Santana et al., Reference Sant'ana, Roque and Eiras2006), as this type of organic detritus creates a profitable environment for bacterial growth. However, specialization to live outdoors and take advantage of oviposition containers that are rich in organic matter may generate an interesting trade off, because outdoor environments can be harsh. For example, highly productive containers, in addition to being profitable for mosquito immatures, may also be desirable environments for conspecifics and heterospecifics (Westby & Juliano, Reference Westby and Juliano2017), which can expose the offspring to both interspecific and intraspecific competition (Juliano et al., Reference Juliano, Lounibos and O'Meara2004; Juliano, Reference Juliano2009); such containers may also be ideal environments for predators, which may threaten the survival of engorged females (Jackson et al., Reference Jackson, Nelson and Sune2005) or offspring survival and fitness (Uitregt et al., Reference Uitregt, Hurst and Wilson2012). Our results for the outdoor oviposition trials show a strong preference for water with organic matter, however this preference was not achieved until the fifth experimental week (fig. 3). One potential explanation is that in the first four weeks, spreading reproductive effort across various containers is more important than searching for those containers holding organic matter. By pooling together weeks 1 to 5 (early) in a factorial design and comparing to weeks 6 to 9 (late) in the presence or absence of organic matter, we showed that organic matter-enriched water attracts A. aegypti females late in the season (fig. 4a). In the late summer, finding containers holding organic matter may be more important for offspring development and may contribute to reproductive success in the following year more than simply spreading eggs.
Alternatively, indoor oviposition may limit the exposure of mosquito females to those negative interactions. Our results show a lack of oviposition preference for CWT or TWT containers indoors (fig. 5), even during the late season (fig. 4b). This result presents an interesting question: why would the A. aegypti oviposition preference for container organic matter concentration differ between indoor and outdoor environments? One potential explanation is that A. aegypti larvae have been reported to inhabit several types of domestic containers such as toilet seats, rain water containers, water boxes (common in Brazilian houses), and potable water tanks (Forattini & Brito, Reference Forattini and Brito2003), and water from these sources typically contains low organic matter concentration (Westphalen et al., Reference Westphalen, Coração and Benetti2016). Despite this, the quantity and diversity of water-holding containers for mosquito offspring development indoors are likely lower than in outdoor environments. The ability of mosquitoes to utilize indoor containers and the lack of preference for water with organic matter may be a product of co-evolution with humans (Juliano & Lounibos, Reference Juliano and Lounibos2016), where oviposition habitat choice indoors may simply reflect opportunistic behavior based on the availability of oviposition sites. However, demonstrating this would require testing a few hypotheses. First, if outdoor and indoor mosquito populations do behave differently with respect to oviposition preferences, this may reflect genetic differences between those populations. For example, Tabachnick & Powell, (Reference Tabachnick and Powell1979) found genetic and behavioral distinctions between sympatric forms of indoor and outdoor (sylvatic) populations of A. aegypti. Those populations also varied in oviposition behavior, with indoor mosquitoes preferentially colonizing man-made containers and sylvatic populations preferentially choosing tree-holes and other plant cavities, which are rich in organic matter content (Cogliatti-Carvalho et al., Reference Cogliatti-Carvalho, Rocha-Pessôa, Nunes-Freitas and Rocha2010; Lima-Camara et al., Reference Lima-Camara, Urbinatti and Chiaravalloti-Neto2016). Such studies support the idea that indoor mosquitoes may behave differently due to lack of exposure to water with high levels of organic matter.
We also cannot rule out the possibility that the same mosquito females could have visited outdoor and indoor containers during the experimental period and can only speculate that the lack of containers with high organic matter indoors combined with easy access to humans for a blood meal could have driven mosquito females to indiscriminately oviposit in the CWT and TWT containers. Food restriction does not seem to strongly impact Aedes larval development compared to other species and genera (e.g., Culex) (Carrieri et al., Reference Carrieri, Bacchi, Bellini and Maini2003; Costanzo et al., Reference Costanzo, Mormann and Juliano2005), indicating that Aedes larvae are well-adjusted to low food levels.
Lastly, it is well-known that Aedes aegypti females exhibit skip oviposition behavior (Colton et al., Reference Colton, Chadee and Severson2003), where eggs are spread among containers located in close proximity to one another. Although we cannot rule out that our results happened only by chance, the fact that females laid proportionally more eggs in TWT containers combined with skip oviposition behavior suggests as preference from containers with organic detritus. Previous evidence suggests that this is possibly stimulated by bacterial products associated with detritus, which indicates a profitable environment for offspring development (Albeny-Simões et al., Reference Albeny-Simões, Murrell, Elliot, Andrade, Lima, Juliano and Vilela2014).
Further investigations of A. aegypti oviposition preferences among man-made containers located inside or outside of residences will improve our understanding of the main behavioral factors contributing to the success of mosquito populations in anthropogenic environments (Hufbauer et al., Reference Hufbauer, Facon, Ravigne, Turgeon, Foucaud, Lee, Rey and Estoup2012). Additional studies are needed to better understand the colonization and oviposition behavior of A. aegypti in both urban and residential environments.
Acknowledgments
CNPq provided financial support for this project through an undergraduate research fellowship to MC and GDC. We thank the homeowners who kindly agreed to host the oviposition traps for the experimental period.