Introduction
Faba bean (Vicia faba L.) is a high-protein, nutritious grain legume crop. Its mixed breeding system and unknown wild progenitor along with its large and complex genome [2n = 2x = 12, haploid genome size ~13 Gbp (Soltis et al., Reference Soltis, Soltis, Bennett and Leitch2003)] are important challenges for faba bean genetic and breeding studies (O'Sullivan and Angra, Reference O'Sullivan and Angra2016).
Bi-parental crosses used to develop F2, recombinant inbred line and backcross populations for genetic studies have been used to map quantitative trait loci for genetic traits of interest in faba bean. However, these types of genetic populations are limited by their genetic recombination level and only two alleles are present at any locus (Singh and Singh, Reference Singh, Singh, Singh and Singh2015). In contrast, multi-parent advanced generation intercross (MAGIC) populations present multiple alleles, resulting in increased recombination and mapping resolution for complex traits (Cavanagh et al., Reference Cavanagh, Morell, Mackay and Powell2008). The multi-parent nature of MAGIC populations increases the intercrossing and shuffling of the genome, which makes them better suited for genetic studies, particularly for faba bean which has limited genomic resources. Multi-parent populations also provide deeper knowledge on genomic structure and improve pre-breeding resources (Huang et al., Reference Huang, Verbyla, Verbyla, Raghavan, Singh, Gaur, Leung, Varshney and Cavanagh2015). They are powerful tools for identifying alleles and loci responsible for economically important traits, especially with the recent availability of affordable high-throughput genotyping platforms and advances in statistical methods of data analysis (Meng et al., Reference Meng, Guo, Ponce, Zhao and Ye2016).
Multi-parent populations have been developed and analysed in various plant species (reviewed in Huang et al., Reference Huang, Verbyla, Verbyla, Raghavan, Singh, Gaur, Leung, Varshney and Cavanagh2015). In faba bean, a multi-parent population derived from 11 European winter bean collection was employed to identify genomic regions governing frost adaptation, using 189 individuals and 156 single nucleotide polymorphism (SNP) markers (Sallam and Martsch, Reference Sallam and Martsch2015).
The current paper introduces a large faba bean population derived from intercrossing four inbred lines that are genetically contrasting for important agro-morphological traits including drought adaptation, seed morphology, seed chemistry and disease resistance. The segregation patterns of Mendelian traits such as pigmentation of stipule spots and flowers at different generations are presented.
Experimental details
Parental line selection
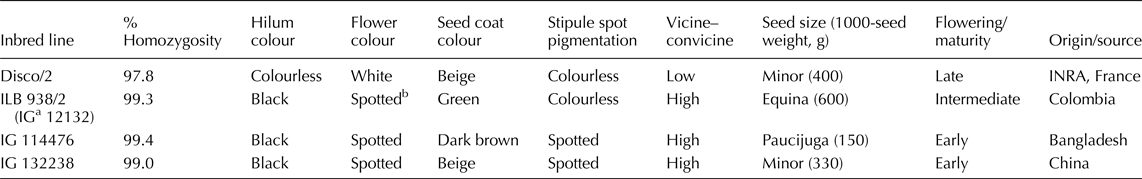
The four faba bean inbred lines used to create the multi-parent population and their morphological and biochemical characteristics of interest are shown in Table 1. More information on potential traits for phenotyping including physiological traits and seed morphology and seed chemistry is presented in online Supplementary Table S1. Each parental line was selfed for three generations to reach a higher level of homozygosity before F1 crosses were made.
Per cent homozygosity, in six key traits and origin of the four faba bean parental inbred lines used in this study

a IG, ICARDA (International Centre for Agricultural Research in the Dry Areas) accession number. More information about accessions can be found at http://www.genesys-pgr.org/.
b Flowers display a dark spot on the wing petals and also dark vein marking on the standard petal (wild type).
INRA, Institut National de la Recherche Agronomique.
Disco/2 is a selection from the zero-tannin cultivar Disco carrying the zt2 gene (Picard, Reference Picard1976; Gutierrez et al., Reference Gutierrez, Avila, Moreno and Torres2008) and low vicine–convicine (vc− gene, Duc et al., Reference Duc, Sixdenier, Lila, Furstoss, Huisman, van der Poel and Liener1989; confirmed in Khamassi et al., Reference Khamassi, Ben Jeddi, Hobbs, Irigoyen, Stoddard, O'Sullivan and Jones2013; Khazaei et al., Reference Khazaei, Purves, Song, Stonehouse, Bett, Stoddard and Vandenberg2017 and Purves et al., Reference Purves, Khazaei and Vandenberg2018). Disco was released in France as a source of combined zero tannin and low v-c (FEVITA type, Duc et al., Reference Duc, Crepon, Marget and Muel2004).
ILB 938/2 (Khazaei et al., Reference Khazaei, Link, Street and Stoddard2018) is a Colombian faba bean accession with high water use efficiency (Link et al., Reference Link, Abdelmula, von Kittlitz, Bruns, Riemer and Stelling1999; Khazaei et al., Reference Khazaei, Street, Bari, Santanen and Stoddard2013, Reference Khazaei, O'Sullivan, Sillanpää and Stoddard2014b) and resistance to chocolate spot (Botrytis fabae, Maalouf et al., Reference Maalouf, Ahmed, Shaaban, Bassam, Nawar, Singh and Amri2016). ILB 938/2 also carries a gene that decouples pigmentation in flowers from pigmentation in stipules (Khazaei et al., Reference Khazaei, O'Sullivan, Sillanpää and Stoddard2014a).
IG 114476 is a Paucijuga-type faba bean with small seeds (1000 seed weight of ~150 g), short stature and highly branched main stem growth habit (personal observation).
IG 132238 is an early maturing faba bean accession (Stoddard et al., Reference Stoddard, Khazaei, Belachew, Bari, Damania, Street, Mackay and Dayanandan2016) from China.
Hybridization
Bi-parental crosses (Disco/2 × ILB 938/2) and (IG 114476 × IG 132238) were made, and then a large number of four-way crosses [(Disco/2 × ILB 938/2) × (IG 114476 × IG 132238)] were made in the insect-proof greenhouse of the Department of Agricultural Sciences, the University of Helsinki, Finland in 2014 (online Supplementary Fig. S1). The population pedigree did not involve a balanced funnel design (using six possible F1 combinations). One thousand two hundred four-way F1 plants were grown and generations were advanced by single-seed descent to the F3 and F4 in the controlled environment conditions facility of the University of Saskatchewan, Canada. In all generations, the growing conditions were maintained in a similar manner. The photoperiod of the growth unit was set to 14/10 h (light/dark). The photosynthetic photon flux density was ~300 µmol/m2/s at the plant canopy level. The temperature was adjusted to 21°C light/15°C dark.
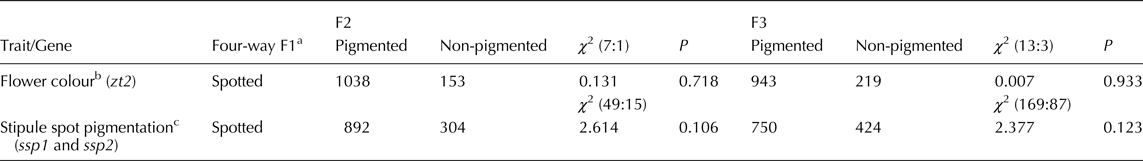
In all three generations, the flower colour and stipule spot pigmentation (SSP) phenotypes were recorded for each plant during population development. The goodness-of-fit of observed segregation ratio to expected ratios for both flower colour and SSP were determined using the standard χ 2 test (R statistics, R Development Core Team, 2016). The expected number of offspring was obtained from the hypothesis of one (flower colour) and two (SSP) unlinked recessive genes.
Parental lines genotyping and simulations
The four inbred parental lines were genotyped using 875 SNP markers developed by Webb et al. (Reference Webb, Cottage, Wood, Khamassi, Hobbs, Gostkiewicz, White, Khazaei, Ali, Street, Stoddard, Maalouf, Ogbonnaya, Link, Thomas and O'Sullivan2016). DNA was extracted from a seedling leaf of a single plant of each parent lines. Nine discs (diameter 5 mm) from healthy, newly expanded leaves of the parental lines were shipped to the LGC Genomics laboratory (LGC Genomics, Beverly, MA, USA) for genomic DNA extraction and SNP genotyping according to the manufacturer's instructions.
GeneDrop (http://www.niab.com/pages/id/376/GeneDrop) was employed for simulations using 14 SNP markers (see online Supplementary Table S3). The number of unique haplotypes of bi-parental population, four-way crosses with simple and multiple funnel schemes were counted as described in Ladejobi et al. (Reference Ladejobi, Elderfield, Gardner, Gaynor, Hickey, Hibberd, Mackay and Bentley2016).
Results and discussion
The four inbred lines used as parents were highly homozygous (Table 1). The genotyping call on parental lines is presented in online Supplementary Table S2. Polymorphic SNPs were 24% when only two bi-parental crosses were considered, but about 47% of SNP markers were polymorphic among lines from four-way crosses. The haplotype diversity of parental lines over 678 mapped SNP markers from the consensus map (Webb et al., Reference Webb, Cottage, Wood, Khamassi, Hobbs, Gostkiewicz, White, Khazaei, Ali, Street, Stoddard, Maalouf, Ogbonnaya, Link, Thomas and O'Sullivan2016) is presented in online Supplementary Table S3. The Medtr2g009270 gene, collinear with the low v-c gene (Khazaei et al., Reference Khazaei, Purves, Song, Stonehouse, Bett, Stoddard and Vandenberg2017), faba bean flanking markers on chromosome 1 both could distinguish Disco/2 as low v-c (online Supplementary Table S3, parental lines phenotyping for v-c was presented in online Supplementary Table S1). The simulation results based on 14 SNP markers revealed the number of haplotypes increased with increasing number of founders (two vs four) and pedigree (four-way cross with simple funnel design vs four-way cross with balanced funnel design) (online Supplementary Table S4). Although the pedigree of this population did not involve a balanced funnel design of a MAGIC four-way cross (Ladejobi et al., Reference Ladejobi, Elderfield, Gardner, Gaynor, Hickey, Hibberd, Mackay and Bentley2016), considerable recombination exists in the population (online Supplementary Table S4).
This population combines important key genes for faba bean breeding such as drought response, flowering date, maturity date, height, and seed morphology (seed size and seed coat colour) and seed chemistry [v-c, L-DOPA (Purves et al., Reference Purves, Zhang, Khazaei and Vandenberg2017), folate and tannin, see online Supplementary Table S1]. These traits make the population suitable for further development of genetic studies and for pre-breeding genetic sources. It also offers the opportunity to develop individuals with the combinations of superior alleles that directly contribute to breeding programmes.
The population was checked for unbiased segregation in each generation. All of the 1200 four-way F1 plants had pigmented stipules and flowers (Table 2). The F2 segregation ratio for zt2 confirmed a monogenic Mendelian inheritance (seven coloured:one colourless), with wild-type flower being dominant to white flower. The F2 segregation ratio for ssp fit 49:15 (pigmented:colourless) at the F2 generation, which fits a model of double-recessive complementary behaviour between two unlinked genes in a four-way cross. In the F3 generation, the segregation pattern fit segregation ratios of 13:3 for zt2 and 169:87 for ssp (Table 2). In the F4 generation, the ratios fit 25:7 for the zt2 gene.
Observed offspring segregation ratios, values of χ 2 test and corresponding P value for studied traits/genes among F1 four-way crosses, F2 and F3 generations

a 1200 plants.
b F4 (spotted 843:white 247, χ 2 (25:7): 0.394, P = 0.530).
c F4 expected ratio is 625:399 (spotted:colourless).
The four parental lines were chosen from different agro-ecological zones, providing a basis for genetic analysis of agro-ecological adaptation. They were representative of four diverse germplasm pools (Mediterranean, subtropical, warm temperate and cool temperate climates) from three continents, from high and low latitudes and altitudes, and representative of both food and feed types. For example, IG 114476 is from the sub-tropical savannah of Bangladesh, ILB 938/2 is from Mediterranean adaptation zone and Disco/2 is from the temperate climate of northern latitudes. IG 132238 is representative of Chinese germplasm which is considered to be distinct from all other faba bean germplasm (Duc et al., Reference Duc, Bao, Baum, Redden, Sadiki, Suso, Vishniakova and Zong2010). The UPGMA cluster analysis results confirmed that the four parental lines are genetically distinct (online Supplementary Fig. S2). In the winter faba bean population (Sallam and Martsch, Reference Sallam and Martsch2015), 11 founders from the UK, France and Germany were distributed in three main groups, but this was not based on their country of origin.
The segregation of flower colour and stipule pigmentation as conferred by the zt2 and ssp genes confirmed the dynamics of the population (Gutierrez et al., Reference Gutierrez, Avila, Moreno and Torres2008; Khazaei et al., Reference Khazaei, O'Sullivan, Sillanpää and Stoddard2014a). Phenotyping for more complex traits such as yield components, physiological and biochemical traits may also be considered when genotyping data become available for this population. Development of molecular markers is an important step toward map-based genetic analysis and can help dissect genotype–phenotype relationships and build genome sequencing assemblies. The current population will be genotyped using 50 K SNP array which will provide a valuable genetic tool for collaborative faba bean research. The plant materials are currently managed and stored at the University of Reading, UK and will be available to other researchers worldwide based on seed quantity requirements.
Supplementary material
The supplementary material for this article can be found at https://doi.org/10.1017/S1479262118000242.
Acknowledgements
The authors acknowledge funding from Emil Aaltonen Foundation (Emil Aaltosen Säätiö), the University of Helsinki, Finland, the Agriculture Development Fund (Government of Saskatchewan, Canada) and the NORFAB project (Protein for the Northern Hemisphere) funded by Innovation Fund Denmark. HK also thanks Markku Tykkyläinen, Sini Lindstrom and Sanna Peltola, technical assistants of the glasshouse of the University of Helsinki for their kind assistance during the experiments in Finland, and Allison Sackville and Michael Miller at the University of Saskatchewan, Canada. Many thanks to Professor Wolfgang Link (Georg-August-University, Göttingen, Germany) for providing the seeds of ILB 938/2 and Disco/2 and Dr Kenneth Street for providing ICARDA germplasm accessions.