


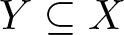

1. Going beyond Buneman Theorem
Trees and associated tree-like objects are very important in mathematics and its applications. There are a variety of invariants which are shown or conjectured to encode a tree structure up to different kinds of equivalences [Reference Aivaliotis, Gordon and Graveman2, Reference Aliste-Prieto, Martin, Wagner and Zamora3, Reference Baez and Otter5, Reference Burghart13, Reference Chaudhary and Gordon17, Reference Dovgoshey and Kostikov23, Reference Dress, Huber and Moulton28, Reference Hendriksen and Kapust48, Reference Dress and Wu31, Reference Liu, Biller, Gould and Colijn55, Reference Loehr and Warrington56, Reference Orellana and Scott58, Reference Pons, Coronado, Hendriksen and Francis61]. Following Buneman [Reference Buneman, Hodson, Kendall and Tautu12], in this paper and its sequel [Reference Qian, Wu and Xie62–Reference Qian, Wu and Xie64], we will be considering how a tree is determined by its split system invariants. After cutting off some tree edges, the leaves of a tree may branch into different groups according to some natural rules. Can we determine the shape of a tree if we have on hand a ‘good’ set of such branchings? To provide a reasonable answer, we must describe the scenario more precisely below.
For any positive integer k, we write  $[k]$ for the set
 $\{1, \ldots,k\}$. Let X be a set. A partition π of X is a family of disjoint subsets
 $X_1,\ldots,X_m$ of X whose union is X. We call the sets
 $X_1,\ldots,X_m$ the parts of π, and we often write π directly as
 $X_1\mid \cdots \mid X_m$. Since there is no ordering of the parts in a partition,
 $Y \mid Z$ is the same as
 $Z\mid Y$. A partition of X into m non-empty parts will be termed an m-partition of X. For any partition π of X and any
 $W\subseteq X$, the restriction of π on W, denoted by
 ${\pi}|_W$, is a partition of W whose parts are the intersections of W with the parts of π. We also write
 $\pi' \subseteq \pi$ to mean that
 $\pi'=\pi|_{W}$ for some set W. An X-split, or a split on X, is simply a partition of X into two parts. A split of X is proper if its two parts are both non-empty; otherwise, it is improper. A family of X-splits is known as an X-split system or a split system on X. An X-split system
 $\mathcal{S}$ is isomorphic to an X′-split system
 $\mathcal{S'}$, denoted by
 $\mathcal{S}\cong \mathcal{S}' $, if there exists a bijection f from X to X′ such that
 $\mathcal{S'}=\{f(Y) \mid f(Z):\ Y \mid Z \in \mathcal{S}\}$.
A graph G is a pair of sets  $\mathrm{V}_G$ and
 $\mathrm{E}_G$ with
 $\mathrm{E}_G\subseteq \binom{\mathrm{V}_G}{2}$; we call
 $\mathrm{V}_G$ its set of vertices and
 $\mathrm{E}_G$ its set of edges. Each edge
 $\{u,v\}$ of a graph is often written as uv. An isomorphism from a graph G to a graph G′ is a bijection f from
 $\mathrm{V}_G$ to
 $ \mathrm{V}_{G'}$ such that
 $uv\in \mathrm{E}_G$ exactly when
 $f(u)f(v)\in \mathrm{E}_{G'}$. We say that G and G′ are isomorphic, designated by
 $G\cong G'$, when there is an isomorphism from G to G′. With a slight abuse of notation, we may sometimes write
 $G=G'$ to mean that
 $G\cong G'$ and write
 $G\in \mathcal{G}$ to mean that G is isomorphic to one element of
 $\mathcal G$.
Let G be a graph. For each  $uv\in \mathrm{E}_G$, we call u and v the endpoints of uv and say that u and v are adjacent in G. For each
 $v\in \mathrm{V}_G$, the set of all vertices adjacent to v in G is denoted by
 $\operatorname{N}_G(v)$ and is named the neighbors of v in G; the size of
 $\operatorname{N}_G(v)$, denoted by
 $\deg_G(v)$, is the degree of v in G. For any non-negative integer
 $\ell$, a path in G of length
 $\ell$ is a sequence of distinct vertices
 $v_0 v_1 \cdots v_\ell$ such that
 $v_0v_1, \ldots, v_{\ell-1}v_\ell\in \mathrm{E}_G$; we do not distinguish this path from its reversal
 $v_\ell v_{\ell-1}\cdots v_0$, and we refer to it as a path between
 $v_0$ and
 $v_\ell$. We call
 $v\in \mathrm{V}_G$ a leaf of G provided
 $\deg_G(v)= 1$, and we reserve the notation
 $\mathrm{L}_G$ for the set of all leaves of G.
A graph is called a tree if there exists a unique path between each pair of its vertices. For a tree T, any element of  $\mathrm{V}_T\setminus \mathrm{L}_T$ is called an inner vertex of T. For any tree T and
 $u,v\in \mathrm{V}_T$, we write
 $T_{u,v}$ for the set of all edges
 $ww'\in \mathrm{E}_T$ such that w and w′ are two adjacent vertices in the unique path between u and v in T. A tree with at least one edge and without any degree-two vertices is called a phylogenetic tree. A binary tree is a phylogenetic tree whose inner vertices are all of degree three. In this paper, we will always assume that a graph has a non-empty and finite vertex set. By this assumption, a graph is a tree if and only if we can remove leaves repeatedly to reach the one-vertex graph, and whenever a phylogenetic tree T is mentioned we should understand that
 $\mathrm{L}_T$ is a finite set of size at least two.
Let X be a finite set with  $|X|\geqslant 2$. A tree T is an X-tree if
 $\{v\in \mathrm{V}_T:\ \deg_T(v)\leq 2\}=X$. Note that, if an X-tree T is phylogenetic, then
 $\mathrm{L}_T=X$. Two X-trees T and T′ are X-isomorphic if there exists a graph isomorphism from T to T′ whose restriction on X is the identity map; we write
 $T\cong_X T'$ to mean that they are X-isomorphic; see Fig. 1.
Phylogenetic [6]-trees T and T′ are isomorphic but not [6]-isomorphic: (A) T and (B) T′

Let T be a tree. For any proper  $\mathrm{L}_T$-split
 $Y\mid Z$, the parsimony score of
 $Y\mid Z$ on T, denoted by
 $\operatorname{PS}(T,Y\mid Z)$, is the minimum positive integer k such that there exists
 $F\in \binom{\mathrm{E}_T}{k}$ which intersects with
 $T_{y,z}$ for every
 $y\in Y$ and
 $z\in Z$ [Reference Fischer36, Reference Forcey38, Reference Semple and Steel66]. The parsimony score of
 $\mathrm{L}_T\mid \emptyset$ is defined to be 0. For any non-negative integer k, we write
 $\mathcal{P}_{T,k}$ for the set of all
 $\mathrm{L}_T$-splits with parsimony score k on T, and name it the score-k split system on T. It is clear that
 $\mathcal{P}_{T,k}$,
 $k\geqslant 0$, are pairwise disjoint. Note that
 $\mathcal{P}_{T,0}$ only contains
 $\mathrm{L}_T \mid \emptyset$ and
 $\mathcal{P}_{T,1}$ is the usual split system considered in phylogenetic combinatorics, namely the one induced by deleting one edge of T.
A split system  $\mathcal{S}$ is compatible provided
 $\prod_{i,j \in [2]}|{Y_i\cap Z_j}|=0$ holds for all
 $Y_1\mid Y_2, Z_1\mid Z_2\in \mathcal{S}$. A split is trivial if one of its parts is a singleton set. Here is the famous split equivalence theorem about score-1 split systems of phylogenetic trees. Note that what Buneman really proved are Theorem 1.1 (1) and (2); but it is not hard to derive Theorem 1.1 (3) as an easy consequence of Theorem 1.1 (2).
Theorem 1.1. (Buneman Theorem [Reference Buneman, Hodson, Kendall and Tautu12])
Let X be a finite set.
(1) An
 $X$-split system
$\mathcal{S}$ is the score-1 split system on a phylogenetic tree if and only if
$\mathcal{S}$ is compatible, does not contain the improper
$X$-split and contains all trivial
$X$-splits.
(2) Two phylogenetic
$X$-trees
$T$ and
$T^{\prime}$ are
$X$-isomorphic if and only if
$\mathcal{P}_{T,1}$ and
$\mathcal{P}_{T',1}$ are equal.(3) Two phylogenetic trees
$T$ and
$T^{\prime}$ are isomorphic if and only if
$\mathcal{P}_{T,1}$ and
$\mathcal{P}_{T',1}$ are isomorphic.


Example 1.2. Let  $\mathrm{K}_{1,3}$,
 $ \mathtt{A}_i$ and
 $\widetilde{\mathtt{A}}_i$,
 $i\in \{-\infty,0\}$, be the trees depicted in Fig. 2, which are pairwise non-isomorphic. Among these five trees, only
 $\mathtt{A}_{-\infty}$ is not a phylogenetic tree. Note that a tree T has
 $\mathcal{P}_{T,2}=\emptyset$ if and only if
 $T\in \{\mathtt{A}_{-\infty}, \widetilde{\mathtt{A}}_{-\infty} , \mathrm{K}_{1,3}\} $. One can also verify that
 $\mathcal{P}_{\mathtt{A}_{0},2}=\mathcal{P}_{\widetilde{\mathtt{A}}_{0},2}=\{Y\mid ([6]\setminus Y):\ Y\in \binom{[6]}{2}\}$; see Lemma 5.1 if you wish to avoid performing the routine calculations yourself. A reader curious about the naming of the graphs in Fig. 2 may refer to
 $\S$ 6.
Two groups of trees with isomorphic score-2 split systems. A)  $\mathtt{A}_{-\infty}$ B)
 $\widetilde{\mathtt{A}}_{-\infty}$ C)
 $\mathrm{K}_{1,3}$ D)
 $\mathtt{A}_0$ E)
 $\widetilde{\mathtt{A}}_0$

There is a significant body of work aimed at deducing results in the same spirit as the Buneman Theorem (Theorem 1.1) [Reference Casanellas and Fernández-Sánchez15, Reference Fischer36, Reference Fischer, van Iersel, Kelk and Scornavacca37, Reference Galashin and Postnikov40, Reference Wilkes71, Reference Hellmuth, Huber, Moulton, Scholz and Stadler44, Reference Wilde and Fischer69, Reference Wilde and Fischer70]. In this paper, we will develop additional variants of Theorem 1.1 (2) and (3); see Theorem 1.3. Corresponding possible variants of Theorem 1.1 (1) are certainly of interest, but so far we have no results to report in that direction.
Theorem 1.3. Let X be a finite set with  $|X|\geqslant 2$, and let T and
 $T'$ be two phylogenetic X-trees.
(1) The tree T is isomorphic to
$\mathtt{A}_0$ or
$\widetilde {\mathtt{A}}_0 $ if and only if
$|X|=6$ and
$\mathcal{P}_{T,2}=\{Y\mid (X\setminus Y):\ Y\in \binom{X}{2}\}$.(2) Assume that
$\{T,T'\}\setminus \{\mathtt{A}_0, \widetilde {\mathtt{A}}_0\}\neq \emptyset$. Then,
$ T \cong_X T' $ if and only if
$ \mathcal{P}_{T,2} = \mathcal{P}_{T',2} $.(3) Assume that
$\{T,T'\}\setminus \{\mathtt{A}_0, \widetilde {\mathtt{A}}_0\}\neq \emptyset$. Then,
$ T \cong T' $ if and only if
$ \mathcal{P}_{T,2} \cong \mathcal{P}_{T',2} $.


Clearly, if two phylogenetic X-trees are both isomorphic to  $\mathtt{A}_0$, then they must be X-isomorphic. However, this does not hold for
 $\widetilde {\mathtt{A}}_0$, as can be seen from Fig. 1. This difference between
 $\widetilde {\mathtt{A}}_0$ and
 $\mathtt{A}_0$ is reflected in the following immediate consequence of Theorem 1.3 (2).
Corollary 1.4. Suppose phylogenetic  $X$-trees
 $T$ and
 $T^{\prime}$ are isomorphic but not
 $X$-isomorphic. If
 $\mathcal{P}_{T,2}=\mathcal{P}_{T',2}$, then both
 $T$ and
 $T^{\prime}$ are isomorphic to
 $\widetilde {\mathtt{A}}_0$.
For any two binary X-trees T and T′, Fischer [Reference Fischer36, Proposition 1] observed that  $\mathcal{P}_{T,2}= \mathcal{P}_{T',2}$ if and only if
 $ T \cong_X T' $. To address general phylogenetic trees, our proof of Theorem 1.3 diverges significantly from her approach in [Reference Fischer36].
Let G be a graph. For any  $A\subseteq \mathrm{V}_G$, the subgraph of G induced by A, designated by
 $G[A]$, is the graph with vertex set A and edge set
 $\mathrm{E}_G \cap \binom{A}{2}$; we use the notation G − A to stand for the subgraph of G induced by
 $\mathrm{V}_G\setminus A$. For any
 $F\subseteq \mathrm{E}_G$, G − F represents the graph with vertex set
 $\mathrm{V}_G$ and edge set
 $\mathrm{E}_G\setminus F$. For a singleton set
 $\{a\}$ contained in either
 $\mathrm{V}_G$ or
 $\mathrm{E}_G$, we write G − a as shorthand for
 $G-\{a\}$. A tree T is a subtree of G if
 $\mathrm{V}_{T}\subseteq \mathrm{V}_G$ and
 $\mathrm{E}_{T}\subseteq \mathrm{E}_G$. For any
 $u,v\in \mathrm{V}_G$, we say that u and v are reachable in G provided there is a path between them in G. This reachability relation on
 $\mathrm{V}_G$ is an equivalence relation; a connected component of G is defined as an equivalence class in this equivalence relation. For any
 $v\in \mathrm{V}_G$, we use
 $\operatorname{C}_G[v]$ to represent the connected component of G containing v. Let T be a tree and take
 $v\in \mathrm{V}_T\setminus \mathrm{L}_T$ with
 $k\doteq \deg_T(v)$. The k-partition
 $X_1\mid \cdots \mid X_k$ of
 $\mathrm{L}_T$, where
 $\{X_1,\ldots, X_k\}=\{\mathrm{L}_T\cap \operatorname{C}_{T-v}[u]:\ u\in \operatorname{N}_T(v)\}$, is denoted by
 $\pi_{T,v}$ and called a one-vertex partition of T.
Our proof of Theorem 1.3 is largely algorithmic. For any given finite set X with  $|X|\geqslant 2$ and any X-split system
 $\mathcal{S}$, our main algorithm, Algorithm 2, as presented in
 $\S$ 5, outputs all phylogenetic X-trees, up to X-isomorphism, whose score-2 split system is exactly
 $\mathcal{S}$. Our Algorithm 2 is based on Algorithm 1, which is introduced in
 $\S$ 3. For any given finite set X, integer
 $k\geqslant 4$, X-split system
 $\mathcal{S}$, and k-partition π of X, Algorithm 1 outputs all phylogenetic X-trees T having π as a one-vertex partition and satisfying
 $\mathcal{S} =\mathcal{P}_{T,2} $. In other words, when a potential phylogenetic tree T with
 $\mathcal{S}= \mathcal{P}_{T,2} $ contains a vertex of degree at least four, Algorithm 1 reconstructs this tree T; see Lemma 3.3. Algorithm 2 essentially consists of two parts: identifying one of three possible markers and executing the three corresponding reduction steps. The so-called markers are three special structures that need to be recognized from the given split system, namely a potential vertex of degree at least five, a potential cherry, and a potential claw; see
 $\S$ 2.1 for precise definitions of cherry and claw, and see Fig. 3 for a depiction of the three markers. Assuming the existence of a phylogenetic tree T with
 $\mathcal{P}_{T,2}=\mathcal{S}$, a sketch of the corresponding reduction steps of Algorithm 2 is roughly as follows:
• If there exists a vertex of degree at least 5 in T, then reconstruct T using Algorithm 1.
• If there is a cherry in T, then we can perform a reduction by deleting cherries; see Lemma 3.1.
• If there is no vertex of degree at least 5 and at most one cherry in T, then T must contain a claw. Consequently, we can reconstruct T using Algorithm 1.
Three markers. A)  $Y_1\mid \cdots \mid Y_{k+2}=\pi_{T,v} $ for some
 $v\in \mathrm{V}_T$ with
 $\deg_T(v)\geqslant 5$. B)
 $\{x,y\}$ is a cherry. C)
 $\{x,y,z\}$ is a claw.

Construct a phylogenetic X-tree from a split system and a k-partition of X

Reconstruct a phylogenetic tree T from  $ \mathcal{P}_{T,2} $

Note that detecting cherry information is straightforward (Corollary 2.7); however, the treatment of the other two types of markers is more involved. In  $\S$ 4.1, we begin with Definitions 4.1 and 4.2, which introduce
 $(k,2)$-sets with respect to a split system and 2-special configurations in a tree, respectively. The main result there, Lemma 4.4, provides a correspondence between
 $(k,2)$-sets and 2-special configurations, helping us extract graph structures of the phylogenetic tree from split system information. In
 $\S$ 4.2, we demonstrate how to identify from
 $\mathcal{P}_{T,2}$ a potential vertex v in T with
 $\deg_T(v)\geqslant 5$ (Lemma 4.13), and, in the event that
 $|{\mathrm{L}_T}|\geqslant 7$ and
 $\max_{v\in \mathrm{V}_T}\deg_T(v)\leq 4$, how to detect a claw (Lemma 4.15).
We organize the proof details of Theorem 1.3 in the next four sections. Section 2 is dedicated to technical preparations. The main results of  $\S$ 3 are Lemma 3.1 and Algorithm 1, where Lemma 3.1 describes the effect of the cherry-deletion operation on the score-2 split system, and Algorithm 1 provides a method to construct a tree T from its score-2 split system or its 2-split system (see
 $\S$ 2 for the definition) when
 $\pi_{T,v}$ is given as input for some
 $v\in \mathrm{V}_T$ with
 $\deg_T(v)\geqslant 4$. Note that Algorithm 1 will also be used in our subsequent work on recovering a tree from its 2-split system [Reference Qian, Wu and Xie62]. In
 $\S$ 4, we develop a method to recognize either a one-vertex partition into at least five non-empty parts or a claw in a tree from its score-2 split system. In
 $\S$ 5, we present Algorithm 2 and provide a concise proof of Theorem 1.3. We conclude this paper by highlighting some further results and open questions related to this line of research in
 $\S$ 6.
2. Preliminaries
2.1. A bit more notations
For a set Y and a singleton set  $Z=\{z\}$, we often write
 $Y\cup Z$ and
 $Y\setminus Z$ as Y + z and Y − z, respectively.
Let G be a graph.
For distinct  $x,y\in \mathrm{L}_G$ and
 $v\in \mathrm{V}_G$, we call
 $\{x,y\}$ a cherry and
 $\{x,y;v\}$ a full cherry of G if
 $\deg_G (v)=3$ and
 $\{x,y\}\subseteq \operatorname{N}_G(v)$. We call
 $\{x,y,z\}\in \binom{\mathrm{L}_G}{3}$ a claw of G provided there exists
 $w\in \mathrm{V}_G$ such that
 $\operatorname{N}_G(w) \cap \mathrm{L}_G=\{x,y,z\}$ and
 $\deg_G(w)=4$. For each integer
 $n\geqslant 3$, the star graph
 $\mathrm{K}_{1,n}$ is a tree on n + 1 vertices in which every two edges share a common endpoint.
We say that  $e\in \mathrm{E}_G$ is incident with
 $v\in \mathrm{V}_G$ in G if v is an endpoint of e, namely
 $v\in e$. The number of connected components of G is denoted by
 $\operatorname{c}(G)$. We refer to G as a connected graph whenever
 $\operatorname{c}(G)\leq 1$. For any
 $U,V\subseteq \mathrm{V}_G$, we say that U and V are reachable to each other in G provided there exist
 $u\in U$ and
 $v\in V$ such that
 $\operatorname{C}_G[u]=\operatorname{C}_G[v]$.
For any  $u,v\in \mathrm{V}_G$, the shortest length of a path between them in G is called the distance between them in G, which is designated by
 $\operatorname{dist}_G(u,v)$. For any non-empty subsets
 $U, W \subseteq \mathrm{V}_G$, the notation
 $\operatorname{dist}_G(U,W)$ represents
 $\min_{u\in U, w\in W}\operatorname{dist}_G(u,w)$, whereas
 $[U,W]_G$ consists of all vertices
 $v\in \mathrm{V}_G \ \text{such that}\ \operatorname{dist}_G(U, v)+\operatorname{dist}_G(v, W)=\operatorname{dist} _G(U,W)$.
For any  $U\subseteq \mathrm{V}_G$, the coboundary of U in G, denoted by
 $\partial_G(U)$, is the set
 $\{uv\in \mathrm{E}_G:\ u\in U, v\in \mathrm{V}_G\setminus U\}$.
2.2. Parsimony score,
$\ell$-split and smallest 2-extension

In this subsection, we introduce two basic concepts for our work:  $\ell$-splits and smallest 2-extensions. In addition, we discuss the parsimony score of a 2-split and establish some basic results about smallest 2-extensions.
In mathematics, parity considerations are often used to associate an invariant to a graph [Reference Backelin and Linusson4, Reference Dress, K. T., Huber and Moulton24, Reference Oum59]. Let us introduce a class of tree-like split systems from this parity perspective. Let T be a tree. For any  $V\subseteq \mathrm{V}_T$ and
 $F\subseteq \mathrm{E}_T$, we define a split
 $\widehat{\mathbf{S}}_{T,F,V}$ on V by requiring
 $u,v\in V$ to fall into the same part of
 $ \widehat{\mathbf{S}}_{T,F,V}$ if and only if
 $|{T_{u,v}\cap F}|$ is an even integer. Given any
 $\mathrm{V}_T$-split
 $U \mid W$, it is clear that
 $\widehat{\mathbf{S}}_{T,F, \mathrm{V}_T }=U \mid W$ if and only if
 $F=\partial_T (U )=\partial_T (W )$. The coboundary map
 $\partial_T$ [Reference Wu72, § 2] indeed induces a natural bijection from the set of all
 $\mathrm{V}_T$-splits to the powerset of
 $\mathrm{E}_T$, both having size
 $2^{|{\mathrm{V}_T}|-1}=2^{|{\mathrm{E}_T}|}$. Take a non-negative integer
 $\ell$. For any
 $V\subseteq \mathrm{V}_T$, we define the split system
 $ \widehat{\mathcal{S}}_{T,\ell,V}$ on V by setting
 \begin{equation*} \widehat{\mathcal{S}}_{T,\ell ,V}\doteq \left\{\widehat{\mathbf{S}}_{T,F,V}:\ F\in \binom{\mathrm{E}_T}{\ell}\right\}.\end{equation*}
For any edge set  $F\subseteq \mathrm{E}_T$, we exploit the shorthand
 $\mathbf{S}_{T,F}$,
 $\mathcal{S}_{T,\ell}$,
 $ \widehat{\mathbf{S}}_{T,F }$ and
 $ \widehat{\mathcal{S}}_{T,\ell }$ for
 $ \widehat{\mathbf{S}}_{T,F,\mathrm{L}_T }$
 $ \widehat{\mathcal{S}}_{T,\ell , \mathrm{L}_T}$,
 $ \widehat{\mathbf{S}}_{T,F,\mathrm{V}_T }$ and
 $ \widehat{\mathcal{S}}_{T,\ell , \mathrm{V}_T}$, respectively. We call
 $\mathcal{S}_{T,\ell}$ the
 $\ell$-split system on T. Clearly,
 $\mathcal{P}_{T,0 }=\mathcal{S}_{T,0 }=\{\mathrm{L}_T\mid \emptyset\}$, and
 $\operatorname{PS}(T,\mathbf{S}_{T,F})\leq \ell$ when
 $F\in \binom{\mathrm{E}_T}{\ell}$.
Example 2.1. Let T be a tree, and let  $F\subseteq \mathrm{E}_G$. Then,
 $\mathbf{S}_{T,F}=\mathrm{L}_T\mid \emptyset$ if and only if
 $F=\partial_T(U)$ for some
 $U\subseteq \mathrm{V}_T\setminus \mathrm{L}_T$.
Lemma 2.2. Let  $T$ be a tree. For every non-negative integer
 $k$, it holds that
 $\mathcal{P}_{T,k }=\mathcal{S}_{T,k }\setminus \left(\bigcup_{i=0}^{k-1}\mathcal{S}_{T,i}\right)$. Therefore, for every
 $\mathrm{L}_T$-split
 $\mathbf{S}$, it holds that
 $\operatorname{PS}(T, \mathbf{S})=\min \{k:\ \mathbf{S}\in \mathcal{S}_{T,k} \}$.
Proof. It is clear that  $\mathcal{P}_{T,0}, \mathcal{P}_{T,1}, \ldots $ are pairwise disjoint. Henceforth, to show that
 $\mathcal{P}_{T,k }=(\bigcup_{i=0}^{k}\mathcal{P}_{T,i})\setminus (\bigcup_{i=0}^{k-1}\mathcal{P}_{T,i})$ is equal to
 $\mathcal{S}_{T,k }\setminus (\bigcup_{i=0}^{k-1}\mathcal{S}_{T,i})=(\bigcup_{i=0}^{k}\mathcal{S}_{T,i})\setminus (\bigcup_{i=0}^{k-1}\mathcal{S}_{T,i})$, we only need to verify that
 $\bigcup_{i=0}^{k}\mathcal{P}_{T,i}=\bigcup_{i=0}^{k}\mathcal{S}_{T,i}$ holds for each non-negative integer k. Since
 $ \bigcup_{i=0}^{k}\mathcal{S}_{T,i} \subseteq \bigcup_{i=0}^{k}\mathcal{P}_{T,i}$ holds trivially, our task reduces to proving that
 $\mathcal{P}_{T,k }\subseteq \mathcal{S}_{T,k } $.
Consider an  $\mathrm{L}_T$-split
 $Y\mid Z\in \mathcal{P}_{T,k}$. By definition, there exists a set
 $F\in \binom{\mathrm{E}_T}{k} $ intersecting with
 $T_{y,z}$ for each
 $y\in Y$ and
 $z\in Z$. Since T is a tree, there are k + 1 connected components
 $V_1,\ldots, V_{k+1}$ in T − F. Denote
 $V_i\cap \mathrm{L}_T$ by
 $\mathrm{L}_i$ for each
 $i\in [k+1]$. Clearly,
 $\mathrm{L}_i\mid \emptyset \subseteq Y\mid Z$ for each
 $i\in [k+1]$. For any
 $f\in F$, say
 $f=u_iu_j$ with
 $u_i\in V_i$ and
 $u_j\in V_j$, from
 $\operatorname{PS}(T,Y\mid Z)=|{F}|$ we derive the existence of
 $y\in Y$ and
 $z\in Z$ such that
 $\{f\}=F\cap T_{y,z}$. This then implies that both
 $\mathrm{L}_i$ and
 $\mathrm{L}_j$ are non-empty and
 \begin{equation}
\mathrm{L}_i\mid \mathrm{L}_j \subseteq Y\mid Z.
\end{equation}
We now construct a tree T′ on  $[k+1]$ such that ij is an edge if and only if
 $\operatorname{dist}_T(V_i,V_j)=1$. Let
 $U\mid W$ be the unique partition of
 $\mathrm{V}_{T'}$ into its two independent sets. From Eq. (1), we infer that
 $\{Y,Z\}=\{\cup_{i\in U}\mathrm{L}_i, \cup_{j\in W}\mathrm{L}_j \}$, and thus
 $Y\mid Z = \mathbf{S}_{T,F} \in \mathcal{S}_{T,k}$, as desired.
Lemma 2.3. Let  $T$ be a tree and
 $e ,e' \in \mathrm{E}_T$. Then
 $\mathbf{S}_{T,\{e,e'\}}$ is improper if and only if
 $e\neq e'$ and
 $\deg_T(w)=2$ for all
 $w\in [e,e']_T$. In particular, if
 $T$ is a phylogenetic tree, then
 $\mathrm{L}_T\mid \emptyset \notin \mathcal{S}_{T,1}\cup \mathcal{S}_{T,2}$.
Proof. Assume that e = uv. Take  $x\in \mathrm{L}_T\cap \operatorname{C}_{T-e }[u]$ and
 $y \in \mathrm{L}_T\cap \operatorname{C}_{T-e }[v] $. Clearly, x and y fall into different parts of
 $\mathbf{S}_{T,\{e\} }$, showing that
 $\mathbf{S}_{T,\{e\} }$ is proper.
If  $e\neq e'$ and
 $\deg_T(w)=2$ for all
 $w\in [e,e']_T$, then
 $\mathbf{S}_{T,\{e,e'\}}$ is surely improper.
It remains to show that  $\mathbf{S}_{T,\{e,e'\}}$ is proper in the case that
 $e\neq e'$ and
 $[e,e']_T$ contains a vertex w with
 $\deg_T(w)\geqslant 3$. We first find
 $x , y \in \mathrm{L}_T$ such that
 $\{e, e'\}\subseteq T_{x , y}$. Thanks to
 $\deg_T(w)\geqslant 3$, we can then pick a vertex
 $w'\in \operatorname{N}_T(w)$ outside the path between x and y in T. Choose
 $z\in \mathrm{L}_T\cap \operatorname{C}_{T-w}[w'] $. One can check that x and z fall into different parts of
 $\mathbf{S}_{T,\{e,e'\}}$, and thus
 $\mathbf{S}_{T,\{e,e'\}}$ is a proper split.
Remark 2.4. Let T be a tree. By Lemma 2.2,  $\mathcal{P}_{T,1}=\mathcal{S}_{T,1}\setminus \mathcal{S}_{T,0}$ and
 $\mathcal{P}_{T,2}=\mathcal{S}_{T,2}\setminus (\mathcal{S}_{T,1}\cup \mathcal{S}_{T,0})$. Recall that
 $\mathcal{S}_{T,0}=\{\mathrm{L}_T\mid \emptyset\}$. Therefore, a further application of Lemma 2.3 shows that
 $\mathcal{P}_{T,1}=\mathcal{S}_{T,1} $, and that, when T is even a phylogenetic tree,
 $\mathcal{P}_{T,2}=\mathcal{S}_{T,2}\setminus \mathcal{S}_{T,1}$.
Let T be a tree. According to Example 2.1, if  $\mathbf{S}_{T,F_1} = \mathbf{S}_{T, F_2} $, then
 $F_1\triangle F_2=\partial_T(U)$ for some
 $U\subseteq \mathrm{V}_T\setminus \mathrm{L}_T$. If
 $|{F_1}|=1$,
 $|{F_2}|=2$, and T is phylogenetic, we can say more about the structure of F 1 and F 2, as shown in Lemma 2.5.
Lemma 2.5. Let  $T$ be a phylogenetic tree. Take
 $ \{e_1,e_2\}\in \binom{\mathrm{E}_T }{2}$ and
 $ e_3 \in \mathrm{E}_T $. Then
 $\mathbf{S}_{T,\{e_1,e_2\}} = \mathbf{S}_{T, \{e_3\}} $ if and only if there exists
 $v\in \mathrm{V}_T$ with
 $\deg_T(v)=3$ such that the three edges of
 $T$ incident with
 $v$ are
 $e_1$,
 $e_2$, and
 $e_3$.
Proof. The backward direction is obvious. We only consider the forward direction.
Assume that  $v_1\in e_1$,
 $v_2\in e_2$ and
 $\operatorname{dist}_T(e_1,e_2)=\operatorname{dist}_T(v_1,v_2)$. Note that v 1 and v 2 must be inner vertices of the phylogenetic tree T. If
 $v_1=v_2$ and
 $\deg_T(v_1)=3$, then it is direct from
 $\mathbf{S}_{T,\{e_1,e_2\}} = \mathbf{S}_{T, \{e_3\}} $ that
 $e_1,e_2$, and e 3 are the three edges incident with v 1 in T, as required. We thus assume that either
 $v_1\neq v_2$ or
 $\deg_T(v_1) \gt 3$, and we aim to derive a contradiction. Our assumption now enables us find
 $w_1,w_2\in \mathrm{V}_T$ such that
 $v_1w_1, v_2w_2\in \mathrm{E}_T\setminus (\{e_1,e_2\}\cup T_{v_1,v_2})$ and
 $v_1w_1\neq v_2w_2$. We can accordingly find
 $x_1,y_1,x_2,y_2\in \mathrm{L}_T$ such that, for each
 $i\in [2]$,
 $e_{3-i}\notin T_{x_i,y_i}\supseteq \{e_i, v_iw_i\}$, thus implying that xi and yi belong to different parts of
 $\mathbf{S}_{T,\{e_1,e_2\}}$. Since
 $ T_{x_1,y_1}$ and
 $ T_{x_2,y_2}$ are disjoint, one of them cannot contain the edge e 3. This contradicts
 $\mathbf{S}_{T,\{e_1,e_2\}} = \mathbf{S}_{T,\{e_3 \}} $.
Corollary 2.6. Let  $T$ be a phylogenetic tree and let
 $\{e_1,e_2\}\in \binom{\mathrm{E}_T}{2}$. Then,
 $\mathbf{S}_{T,\{e_1,e_2\}}\notin \mathcal{P}_{T,2}$ if and only if
 $e_1$ and
 $e_2$ share a common endpoint
 $v$ with
 $\deg_T(v)=3$.
Proof. By Remark 2.4,  $\mathbf{S}_{T,\{e_1,e_2\}}\notin \mathcal{P}_{T,2}$ if and only if there exists
 $e_3\in \mathrm{E}_T $ such that
 $\mathbf{S}_{T,\{e_1,e_2\}} = \mathbf{S}_{T, \{e_3\}} $. It follows from Lemma 2.5 that the latter condition is further equivalent to the condition that e 1 and e 2 share a common endpoint v with
 $\deg_T(v)=3$.
Corollary 2.7. Let  $T$ be a phylogenetic tree with at least three leaves and
 $\{x,y\} \in \binom{\mathrm{L}_T}{2}$. Then
 $ \{x,y\}\mid (\mathrm{L}_T\setminus \{x,y\}) \notin \mathcal{P}_{T,2} $ if and only if
 $\{x,y\}$ is a cherry of
 $T$.
Proof. Let e 1 and e 2 be the edges incident with x and y in T, respectively. Note that  $\{x,y\}\mid (\mathrm{L}_T\setminus \{x,y\})=\mathbf{S}_{T,\{e_1,e_2\}}$. The result now follows directly from Corollary 2.6.
Let T be a tree and let F be a set. We adopt the convention that  $\mathbf{S}_{T,F}$ denotes
 $\mathbf{S}_{T,F\cap \mathrm{E}_{T}}$.
Lemma 2.8. Let  $T$ be a tree and let
 $\tilde{T}$ be a subtree of
 $T$. If
 $\mathrm{L}_{\tilde{T}}\subseteq \mathrm{L}_T$, then
 $\mathbf{S}_{\tilde{T}, F }=\mathbf{S}_{T,F}|_{\mathrm{L}_{\tilde{T}}}$.
Proof. Take  $x,y\in \mathrm{L}_{\tilde{T}}\subseteq \mathrm{L}_T$. Clearly, we have
 $T_{x,y}=\tilde{T}_{x,y}$. Therefore, x and y belong to the same part of
 $\mathbf{S}_{\tilde{T},F }$ if and only if they belong to the same part of
 $\mathbf{S}_{T,F }$.
Lemma 2.9. Let  $T$ be a phylogenetic tree and let
 $w_0\in \mathrm{V}_T$. Assume that
 $ \deg_T(w_0)=k$ and
 $\operatorname{N}_T(w_0)\doteq \{w_1,\ldots,w_k\}$. For each
 $j\in [k]$, let
 $V_j\doteq \operatorname{C}_{T-w_0}[w_j]$ and
 $Y_j\doteq \mathrm{L}_T\cap V_j$. Assume that
 $Y \mid Z =\mathbf{S}_{T,\{e_1,e_2\}}$ for some
 $e_1,e_2\in \mathrm{E}_T$ and
 $Y_i\subsetneq Y$ for some
 $i\in [k]$. If
 $|{\{p\in [k]:\ Z\cap Y_p\neq \emptyset \}}|\geqslant 3$, then
 $e_1\neq e_2$ and
 $w_0w_i\in \{e_1,e_2\}$.
Proof. Let us write T′ for the tree  $T[V_i+w_0]$. Take
 $y_i\in Y_i$ and
 $y\in Y\setminus Y_i$. Considering that
 $Z\cap Y_i\subseteq Z\cap Y=\emptyset$ and
 $|{\{p\in [k]:\ Z\cap Y_p\neq \emptyset \}}|\geqslant 3$, we may assume that
 $i\geqslant 4$ and
 $Z\cap Y_j\neq \emptyset$ for all
 $j\in [3]$. This implies the existence of
 $y_j\in Y_j$ for each
 $j\in [3]$ such that
 $|{T_{y_j,y_i}\cap \{e_1,e_2\}}|=1$. Since
 $T_{y_j,w_0}$,
 $j\in [3]$, are three disjoint edge sets, the pigeonhole principle tells us that
 $\{e_1,e_2\}\cap \mathrm{E}_{T'}\neq \emptyset$. For each
 $z\in Z$,
 $\{e_1,e_2\}\cap T_{y,z}$ is a singleton set. As
 $T_{y,z}\cap \mathrm{E}_{T'}=\emptyset$, we see that
 $\{e_1,e_2\}\setminus \mathrm{E}_{T'}\neq \emptyset$. To sum up, we have
 $|{\{e_1,e_2\}\cap \mathrm{E}_{T'}}|=|{\{e_1,e_2\}\setminus \mathrm{E}_{T'}}|=1$, which means that
 $e_1\neq e_2$. Assume that
 $\{e_1\}= \{e_1,e_2\}\cap \mathrm{E}_{T'} $. If
 $V_i=\{w_i\}$, then clearly
 $e_1=w_0w_i$. If
 $|{V_i}|\geqslant 2$, then, applying Lemma 2.8 for
 $F=\{e_1,e_2\}$ and
 $\tilde{T}=T[V_i]$, we find that
 $\mathbf{S}_{T[V_i], \{e_1\} } =Y_i\mid \emptyset$. In view of Lemma 2.3, we now conclude that
 $ e_1 \notin \mathrm{E}_{T[V_i]}$, i.e.,
 $e_1=w_0w_i$.
Let T be a tree. For any  $\mathrm{L}_T$-split S, the full
 $\ell$-split system of T induced by S is defined as
 $\{\widehat{\mathbf{S}} \in \widehat{\mathcal{S}}_{T,\ell}: \ \mathbf{S} = \widehat{\mathbf{S}}|_{\mathrm{L}_T} \}$.
Lemma 2.10. Let  $T$ be a phylogenetic tree and let
 $\mathbf{S} \in \mathcal{S}_{T,2}$. Then the full
 $2$-split system of
 $T$ induced by
 $\mathbf{S}$ is compatible.
Proof. Let  $\mathbf{S} =Y \mid Z \in \mathcal{S}_{T,2}$. Take
 $\{e_1,e_2\}, \{e'_1,e'_2\} \in \binom{\mathrm{E}_T}{2}$ such that
 $ U\mid W=\widehat{\mathbf{S}}_{T,\{e_1,e_2\}}$ and
 $ U'\mid W'=\widehat{\mathbf{S}}_{T,\{e'_1,e'_2\}}$ are two splits satisfying
 $Y=U\cap \mathrm{L}_T=U'\cap \mathrm{L}_T$. We aim to show that either
 $U\subseteq U'$ or
 $W\subseteq W'$. Due to the symmetry between Y and Z as well as the symmetry between
 $ U\mid W$ and
 $ U'\mid W'$, we may assume that
 $\operatorname{c}(T[U])=1$,
 $\operatorname{c}(T[W])=2$ and W 1 and W 2 are the two connected components of
 $T[W]$. For each
 $i\in [2]$, take
 $z_i\in Z\cap W_i$ and let
 $\{w_i\}=W_i\cap e_i$. The scenario we now encounter is depicted in Fig. 4.
Edge boundary of size two in a tree.

Since T is a phylogenetic tree, we have  $\mathrm{L}_{T[W_1]}\cup \mathrm{L}_{T[W_2]}\subseteq \mathrm{L}_T$. Accordingly, as
 $(U\mid W)|_{\mathrm{L}_T}=(U'\mid W')|_{\mathrm{L}_T}=Y\mid Z$, Lemmas 2.3 and 2.8 tell us that, for each
 $i\in [2]$,
 $\mathrm{E}_{T[W_i]}\cap \{e_1', e_2'\}$ cannot be a singleton set. Without loss of generality, we distinguish the following two cases.
CASE 1.  $\{e_1',e_2'\}\subseteq \mathrm{E}_{T[W_1]}$.
This forces  $U'\supseteq U\cup W_2\supseteq U$.
CASE 2.  $\{e_1',e_2'\}\cap \mathrm{E}_{T[W]}=\emptyset$.
Since  $\widehat{\mathbf{S}}_{T,\{e'_1,e'_2\}}|_{\mathrm{L}_T}=(U'\mid W')|_{\mathrm{L}_T}=Y\mid Z$, we know that
 $T_{z_1,z_2}\cap \{e_1', e_2'\}$ contains zero or two elements. Given that
 $\{e_1',e_2'\}\cap \mathrm{E}_{T[W]}=\emptyset$, it follows that
 $T_{w_1,w_2}\cap \{e_1', e_2'\}$ has size zero or two. This demonstrates that
 $W'\supseteq W$, as required.
Let T be a phylogenetic tree. Let Y be a subset of  $ \mathrm{L}_T$ such that
 $Y \mid (\mathrm{L}_T\setminus Y)\in \mathcal{S}_{T,2}$. Lemma 2.10 guarantees the existence of a unique inclusion-minimal element in
 $\{U\subseteq \mathrm{V}_T:\ U\mid (\mathrm{V}_T\setminus U)\in \widehat{\mathcal{S}}_{T,2}, Y=U\cap \mathrm{L}_T\}$. We denote this element by
 $\mathrm{Ext}_{T,Y}$ and call it the smallest 2-extension of Y in T. For a subset Z of
 $ \mathrm{L}_T$ such that
 $Z \mid (\mathrm{L}_T\setminus Z)\in \mathcal{P}_{T,2}$, we know from Lemma 2.2 that
 $Z \mid (\mathrm{L}_T\setminus Z)\in \mathcal{S}_{T,2}$ and thus it makes sense to talk about
 $\mathrm{Ext}_{T,Z}$.
Lemma 2.11. Let T be a phylogenetic tree. Consider  $\{v_1u_1,v_2u_2\}\in \binom{\mathrm{E}_T}{2}$ such that
 $W\mid (\mathrm{V}_T\setminus W)=\widehat{\mathbf{S}}_{T,\{v_1u_1,v_2u_2\}}$ and
 $\{v_1,v_2\}\subseteq W$. If
 $Y=W\cap \mathrm{L}_T$ and
 \begin{equation}
\max\{\deg_T(v_1), \deg_T(v_2)\} +\operatorname{dist}_T(v_1,v_2) \geqslant 5, \end{equation}
then W coincides with  $\mathrm{Ext}_{T,Y}$, the smallest 2-extension of Y in T.
Proof. For each  $i\in [2]$, let
 $T_i=T[\operatorname{C}_{T[W]}[v_i]]$. It is direct from definition that
 $Y\mid (\mathrm{L}_T\setminus Y)=\mathbf{S}_{T,\{v_1u_1,v_2u_2\}}\in \mathcal{S}_{T,2}$ and
 $\mathrm{Ext}_{T,Y}\subseteq W$. The latter implies that
 $\partial_T(\mathrm{Ext}_{T,Y})\subseteq \mathrm{E}_{T[W]}\cup \{v_1u_1,v_2u_2\}= \mathrm{E}_{T_1} \cup \mathrm{E}_{T_2} \cup \{v_1u_1,v_2u_2\} $. Let
 $\partial_T(\mathrm{Ext}_{T,Y})= \{e_1,e_2\}\in \binom{\mathrm{E}_T}{2}$. By symmetry, it suffices to verify that
 $E=\emptyset$, where
 $E\doteq \{e_1,e_2\}\cap \mathrm{E}_{T_1}$.
If  $v_1=v_2$, then
 $\deg_{T_1}(v_1)=\deg_T(v_1)-2 $, and hence, by Eq. (2),
 \begin{equation}
\deg_{T_1}(v_1)\geqslant 5-2=3.
\end{equation}
If  $v_1\neq v_2$, then
 $\deg_{T_1}(v_1)=\deg_T(v_1)-1 \neq 1 $. If
 $v_1\neq v_2$ and
 $v_2\in \mathrm{V}_{T_1}$, we have
 $\deg_{T_1}(v_2)=\deg_T(v_2)-1\neq 1 $. These observations imply that
 $\mathrm{L}_{T_1}\subseteq Y$. Thus, we can apply Lemma 2.8 to get that
 $ \mathbf{S}_{T_1,E} =\mathbf{S}_{T,\{e_1,e_2\}}|_{\mathrm{L}_{T_1}} $ is an improper split. Accordingly, Lemma 2.3 tells us that either
 $E=\emptyset$, or
 $|{E}|=2$ and
 $\deg_{T_1}(w)=2$ for all
 $w\in [e_1,e_2]_{T_1}$. Assume, for the sake of contradiction, that the second possibility happens. Since
 $\deg_{T_1}(w)\neq 2$ for all
 $w\in \mathrm{V}_{T_1}\setminus \{v_1,v_2\}$, we know that
 $\emptyset \neq [e_1,e_2]_{T_1}\subseteq \{v_1,v_2\}$, and hence
 $2\in \{\deg_{T_1}(v_1), \deg_{T_1}(v_2)\}$. By virtue of Eq. (3), one of
 $v_1,v_2$ having degree two forces
 $v_1\neq v_2$. We thus have two cases to consider: 1)
 $[e_1,e_2]_{T_1}=\{v_1,v_2\}$ is of size two; 2)
 $[e_1,e_2]_{T_1}=\{v_i\}\subsetneq \{v_1,v_2\}$ for some
 $i\in [2]$. For case 1), we find that
 $v_1v_2\in \mathrm{E}_T$ and
 $\deg_T(v_1)=\deg_T(v_2)=3$. It follows that
 $\max\{\deg_T(v_1), \deg_T(v_2)\} +\operatorname{dist}_T(v_1,v_2)=4$, violating Eq. (2), as desired. For case 2), we have
 $\deg_T(v_i)=\deg_{T_1}(v_i)+1=3$ and hence
 $\{e\in \mathrm{E}_T:\ v_i\in e\}=\{e_1,e_2,v_iu_i\}$. It follows that
 $\mathbf{S}_{T,\{v_1u_1,v_2u_2\}}=Y\mid (\mathrm{L}_T\setminus Y)=\mathbf{S}_{T,\{e_1,e_2\}}=\mathbf{S}_{T,\{v_iu_i\}}$, which contradicts Lemma 2.5.
Example 2.12. Let T be the tree drawn in Fig. 5. Then,  $\mathrm{Ext}_{T,\{1,2,3,5\}} = \{1,2,3,5,v\} $ and
 $ \mathrm{Ext}_{T,\{1,2,5\}} = \{1,2,5,v,u\} $. This shows that
 $ Y \subseteq Y' $ does not necessarily imply
 $ \mathrm{Ext}_{T,Y} \subseteq \mathrm{Ext}_{T,Y'} $.
A tree with five leaves.

3. Tree-reduction via cherry and tree-growing from non-cherry markers
Lemma 3.1 is a simple result used to handle cherry markers. Based on Lemma 3.1, our main algorithm, Algorithm 2, can reduce the problem of reconstructing a phylogenetic tree T from  $\mathcal{P}_{T,2}$ to the case where T has at most one cherry. In Algorithm 2, after identifying from split system information either a vertex of degree at least five or a claw in the potential phylogenetic tree, we need to extract information from the given split system to grow the entire tree from these two non-cherry local markers. For this purpose, this section presents Algorithm 1 and demonstrates its usefulness in Lemma 3.3. To prove Lemma 3.3, it is necessary to first establish Lemma 3.2.
Lemma 3.1. Let T be a phylogenetic tree with at least four leaves. If  $\{x_1,x_2; v\}$ is a full cherry of T, then
 $\mathcal{P}_{T-\{x_1,x_2\},2} =\bigl\{(Y+v)\mid Z:\ (Y\cup \{x_1,x_2\})\mid Z \in \mathcal{P}_{T ,2}, Y\cup Z = \mathrm{L}_T\setminus \{x_1,x_2\} \bigr\}$.
Proof. Let Y and Z be disjoint subsets of  $\mathrm{L}_T\setminus \{x_1,x_2\}$ and let
 $T'=T-\{x_1,x_2\}$. Note that T′ is a phylogenetic tree with
 $\mathrm{L}_{T'}=(\mathrm{L}_T\setminus \{x_1,x_2\})+v$ and
 $\mathrm{E}_{T'}= \mathrm{E}_T\setminus \{x_1v,x_2v\}$.
Suppose  $(Y+v)\mid Z \in \mathcal{P}_{T',2}$. By Lemma 2.2, there exists
 $\{e_1,e_2\}\in \binom{\mathrm{E}_{T'}}{2} $ such that
 $(Y+v)\mid Z=\mathbf{S}_{T',\{e_1,e_2\}}\in\mathcal{P}_{T',2}$. It follows from Corollary 2.6 that e 1 and e 2 do not share any common endpoint of degree three in T′. This indicates that
 $e_1,e_2\in \mathrm{E}_T$ do not share a common endpoint of degree three in T, and hence, by Corollary 2.6 again,
 $\mathbf{S}_{T,\{e_1,e_2\}}\in \mathcal{P}_{T,2}$. Since
 $e_1,e_2\notin \{x_1v,x_2v\}$, for every
 $x\in Y \cup Z$ and
 $i\in [2]$,
 \begin{equation*} T_{x,x_i}\cap \{e_1,e_2\}=(T_{x,v}\cup \{x_iv\})\cap \{e_1,e_2\}=T_{x,v}\cap \{e_1,e_2\}=(T')_{x,v}\cap \{e_1,e_2\} .\end{equation*}
Thus,  $ (Y\cup \{x_1,x_2\})\mid Z = \mathbf{S}_{T,\{e_1,e_2\}}\in \mathcal{P}_{T,2} $.
Suppose  $(Y\cup \{x_1,x_2\})\mid Z \in \mathcal{P}_{T ,2}$. By Lemma 2.2, there exists a set
 $\{e,e'\}\in \binom{\mathrm{E}_T}{2}$ such that
 $(Y\cup \{x_1,x_2\})\mid Z=\mathbf{S}_{T,\{e,e'\}}\in \mathcal{P}_{T ,2}$. From Corollary 2.6, it follows that e and e′ do not share any common endpoint of degree three in T. Because
 $|{T_{x_1,x_2}\cap \{e,e'\}}|$ is even and
 $x_1v,x_2v$ share a common endpoint of degree three in T, it holds that
 $\{e,e'\}\cap \{x_1v,x_2v\} =\emptyset$. In other words,
 $e,e'\in \mathrm{E}_{T'}$. Noting that
 $|{T'_{x,v}\cap \{e,e'\}}|=|{T_{x,v} \cap \{e,e'\}}|=|{T_{x,x_i}\cap \{e,e'\}}|$ for every
 $x\in Y \cup Z$ and
 $i\in [2]$, we conclude that
 $\mathbf{S}_{T', \{e,e'\}}=(Y+v)\mid Z$. Recall that e and e′ do not share any common endpoint of degree three in T, and hence in T′. Consequently, it follows from Corollary 2.6 that
 $(Y+v)\mid Z\in \mathcal{P}_{T',2}$.
Lemma 3.2. Let T be a phylogenetic tree and take  $v_0\in \mathrm{V}_T$ with
 $\deg_T(v_0)=k\geqslant 4$. Suppose
 $\operatorname{N}_T(v_0)=\{v_1,\ldots,v_k\}$. For every
 $\ell\in [k]$, we denote by
 $Y_\ell$ the set
 $\mathrm{L}_T\cap \operatorname{C}_{T-v_0}[v_\ell]$ and by
 $T_\ell$ the tree
 $ T[\operatorname{C}_{T-v_0}[v_\ell]+v_0]$. For every
 $\{i,j\}\in \binom{[k]}{2}$, it holds that
 $\mathcal{P}_{T_i,1} =\mathcal{S}_{i,j} = \mathcal{S}_{i,j}'$, where
 $\mathcal{S}_{i,j} \doteq \{Y' \mid ((Y_i \setminus Y') + v_0):\ \emptyset \neq Y' \subseteq Y_i, (Y' \cup Y_j) \mid (\mathrm{L}_T \setminus (Y' \cup Y_j)) \in \mathcal{P}_{T,2} \}$ and
 $\mathcal{S}_{i,j}' \doteq \{Y' \mid ((Y_i \setminus Y') + v_0):\ \emptyset \neq Y' \subseteq Y_i, (Y' \cup Y_j) \mid (\mathrm{L}_T \setminus (Y' \cup Y_j)) \in \mathcal{S}_{T,2} \}$.
Proof. From Remark 2.4 we know that  $\mathcal{P}_{T_i,1}=\mathcal{S}_{T_i,1}$ and
 $\mathcal{P}_{T,2}\subseteq\mathcal{S}_{T,2}$. Henceforth, we only need to prove that
 $\mathcal{S}_{T_i,1}\subseteq \mathcal{S}_{i,j}$ and
 $ \mathcal{S}_{i,j}'\subseteq \mathcal{S}_{T_i,1}$.
Take an element from  $\mathcal{S}_{T_i,1}$, say
 $Y' \mid ((Y_i \setminus Y')+v_0)=\mathbf{S}_{T_i,\{e\}}$ for some
 $e\in \mathrm{E}_{T_i}$. First, it follows from Lemma 2.3 that
 $\emptyset \neq Y' \subseteq Y_i$. We next observe that
 $\mathbf{S}_{T,\{e,v_0v_j\}}=(Y' \cup Y_j) \mid (\mathrm{L}_T \setminus (Y' \cup Y_j))$ and the only possible common endpoint of e and
 $v_0v_j$ is v 0. Due to
 $\deg_T(v_0)\geqslant 4$, Corollary 2.6 claims that
 $\mathbf{S}_{T,\{e,v_0v_j\}}\in \mathcal{P}_{T,2} $. This completes the proof of
 $\mathcal{S}_{T_i,1}\subseteq \mathcal{S}_{i,j}$.
Take a set Y′ such that  $\mathbf{S}\doteq Y' \mid ((Y_i \setminus Y') + v_0)\in \mathcal{S}_{i,j}' $. Assume that
 $ (Y' \cup Y_j) \mid (\mathrm{L}_T \setminus (Y' \cup Y_j))=\mathbf{S}_{T,\{e_1,e_2\}} $ for some
 $\{e_1, e_2\}\in \binom{\mathrm{E}_T}{2}$. We need to verify that
 $Y' \mid ((Y_i \setminus Y')+v_0)\in \mathcal{S}_{T_i,1}$. If
 $Y'=Y_i$, then
 $\mathbf{S}=\mathbf{S}_{T_i,\{v_0v_i\}} \in \mathcal{S}_{T_i,1}$. Now assume that
 $\emptyset \neq Y'\subsetneq Y_i$. Since
 $k\geqslant 4$, there are at least three components of
 $T-v_0$ that intersect with
 $ \mathrm{L}_T \setminus (Y' \cup Y_j)$. Applying Lemma 2.9 for
 $Y\doteq Y' \cup Y_j$ and
 $Z\doteq \mathrm{L}_T \setminus (Y' \cup Y_j)$ yields that
 $e_t=v_0v_j$ for some
 $t\in [2]$. By Lemma 2.8,
 $\mathbf{S}_{T_i-v_0,\{e_{3-t}\}}=\mathbf{S}_{T,\{e_1,e_2\}}|_{Y_i}=Y'\mid (Y_i\setminus Y')$. Since
 $Y'\mid (Y_i\setminus Y')$ is proper, we deduce that
 $e_{3-t}\in \mathrm{E}_{T_i}$. Take a leaf
 $y\in \mathrm{L}_T\setminus (Y_i\cup Y_j)$. Then for every
 $x\in Y_i$,
 $(T_i)_{x,v_0}\cap \{e_{3-t} \}=T_{x,y}\cap \{e_1,e_2\}$. Consequently,
 $\mathbf{S} = \mathbf{S}_{T_i,\{e_{3-t}\}} \in \mathcal{S}_{T_i,1}$, as desired.
Lemma 3.3. Let  $ \mathcal{S} $ be a split system on a finite set X and let π be a k-partition of X, where
 $ k \geqslant 4 $. Up to X-isomorphism, there exists at most one phylogenetic X-tree T such that
 $\mathcal{S} \in \{\mathcal{S}_{T,2}, \mathcal{P}_{T,2}\} $ and π is a one-vertex partition of T. If such a phylogenetic X-tree T exists, then, given the inputs
 $X, \mathcal{S}$, and π, the output of Algorithm 1 is the X-tree T.
Proof. Assume that T is a phylogenetic X-tree such that  $\mathcal{S} \in \{\mathcal{S}_{T,2}, \mathcal{P}_{T,2}\} $ and π is a one-vertex partition of T. Let
 $\pi=Y_1\mid \cdots\mid Y_k=\pi_{T,v_0}$ for some
 $v_0\in \mathrm{V}_T\setminus \mathrm{L}_T$. We show that, given the inputs
 $\mathcal{S}$ and π, Algorithm 1 outputs T up to X-isomorphism. For every
 $ i \in [k]$, let Ti be the unique subtree of T with
 $ \mathrm{L}_{T_i} = Y_i + v_0 $; and let
 $ \mathcal{S}_i $ be the split system defined in Line 4 of Algorithm 1. By Lemma 3.2, we have
 $ \mathcal{S}_i = \mathcal{P}_{T_i,1} $ for every
 $ i \in [k] $. According to Theorem 1.1 (2), Ti can be uniquely recovered from
 $ \mathcal{S}_i $ for every
 $ i \in [k] $, as performed in Lines 5 to 9 of Algorithm 1. The construction of T from
 $ T_1,\dots,T_k $ is straightforward; see Line 11 of Algorithm 1.
Note that Algorithm 1 outputs at most one phylogenetic X-tree. Thus, up to X-isomorphism, there is at most one phylogenetic X-tree T satisfying the two required conditions, which completes the proof.
4. Recognize a one-vertex partition into at least five parts or a claw
Let T be a phylogenetic tree. We have Corollary 2.7 as a simple tool to identify a cherry of T from  $\mathcal{P}_{T,2}$. However, locating the other two types of markers in T from
 $\mathcal{P}_{T,2}$ is less straightforward. Section 4.1 establishes a correspondence between the so-called
 $(k,2)$-set with respect to
 $\mathcal{P}_{T,2}$ and five types of 2-special configurations in the tree T; see Definitions 4.1, 4.2 and Lemma 4.4. We continue in
 $\S$ 4.2 to use this correspondence to find the other two markers. Note that every vertex of degree at least five in T must show up in some 2-special configuration of type A. By encoding type-A 2-special configurations via split system information in Lemma 4.13, we can identify those large-degree vertex markers. Under some mild assumptions, Lemma 4.15 shows how to find a claw from the given split system input. In fact, as demonstrated in the proof of Lemma 4.15, each claw of T is embedded in some 2-special configuration of type E associated with T. Although we cannot directly identify all type-E 2-special configurations from
 $\mathcal{P}_{T,2}$, this connection with type E enables us to find all claw markers.
4.1. (k,2)-set and 2-special configuration
Definition 4.1 (
$(k,\ell)$-set)

Let X be a non-empty finite set, and let  $k,\ell$ be positive integers such that
 $\ell\leq k \leq |X|$. If a set family
 $\mathcal{F}$ equals
 $\bigl\{\bigcup_{i\in I}X_i:\ I\in \binom{[k]}{\ell} \bigr\}$ for some k-partition
 $\pi=X_1\mid \cdots \mid X_k$ of X, then
 $\mathcal{F}$ is called a
 $(k,\ell)$-hypergraph on X and denoted by
 $\operatorname{\mathcal{H}}_{\pi, \ell}$. Let
 $\mathcal{S}$ be an X-split system. For every
 $ Y \subseteq X$, let
 $ \Gamma_{\mathcal{S}}(Y) $ stand for the set of inclusion-maximal elements of
 $ \{Z\subsetneq Y :\ Z \mid (X \setminus Z) \in \mathcal{S}\} $. We say that
 $ Y\subseteq X $ is a
 $(k,\ell)$-set with respect to
 $ \mathcal{S} $ if
 $ Y \mid (X \setminus Y) \in \mathcal{S} $ and
 $ \Gamma_{\mathcal{S}}(Y) $ is a
 $(k,\ell)$-hypergraph on Y. The reader may verify that there is no (k, k)-set with respect to
 $\mathcal{S}$.
For any phylogenetic tree T with a vertex v satisfying  $\deg_T(v)=k+2\geqslant 5$ and
 $\operatorname{N}_T(v)=\{v_1,\ldots,v_{k+2}\}$, observe that
 $ \mathrm{L}_T \cap (\bigcup_{i\in [k]}\operatorname{C}_{T-v}[v_i])$ is a
 $(k,2)$-set with respect to
 $\mathcal{P}_{T,2}$. Additional
 $(k,2)$-sets associated with
 $\mathcal{P}_{T,2}$ are described in Lemma 4.4. To introduce Lemma 4.4, the key lemma in our work, one more definition is required.
Definition 4.2 (2-special configuration)
Suppose T is a phylogenetic tree and  $Y\mid (\mathrm{L}_T\setminus Y)\in \mathcal{S}_{T,2}$. Assume that
 $\partial_T(\mathrm{Ext}_{T,Y}) =\{v_1u_1,v_2u_2\} \in \binom{\mathrm{E}_T}{2}$,
 $\{v_1,v_2\}\subseteq \mathrm{Ext}_{T,Y}$, and
 $\deg_T(v_1)\geqslant \deg_T(v_2)$. Denote
 $\operatorname{c}(T[\mathrm{Ext}_{T,Y}]-(\{v_1,v_2\}\setminus \mathrm{L}_T))$ by
 $\phi_T(Y)$. We call (T, Y) a 2-special configuration whenever one of the following five conditions holds.
(A)
$v_1=v_2$ and
$\deg_T(v_1)\geqslant 5$. See Fig. 6(A).(B)
$v_1v_2\in \mathrm{E}_T$ and
$ \deg_T(v_1)=\deg_T(v_2)=4$. See Fig. 6(B).(C)
$v_1v_2\in \mathrm{E}_T$ and
$ \deg_T(v_1)-1 = \deg_T(v_2) = 3$. See Fig. 6(C).(D)
$T[W]$ is connected,
$ \operatorname{dist}_T(v_1,v_2) \gt 1$ and
$ \deg_T(v_1)=\deg_T(v_2)=3$. See Fig. 6(D).(E)
$ |{Y}|=\deg_T(v_1)=4$,
$\deg_T(v_2)=1$, and either
$u_1\neq u_2$ or
$ \deg_T(u_1) \geqslant 4 $. See Fig. 6(E).


Five types of 2-special configurations (T, Y). Each Yi represents a subset of  $X=\mathrm{L}_T$ within a corresponding subtree. See Definition 4.2. A)
 $\phi_T(Y)=k$ B)
 $\phi_T(Y)=4$ C)
 $\phi_T(Y)=3$ D)
 $\phi_T(Y)=3$ E)
 $\phi_T(Y)=4$

For any 2-special configuration (T, Y), we say that its type is A, B, C, D, or E if the corresponding condition (A), (B), (C), (D), or (E) holds, respectively. When (T, Y) is a 2-special configuration of type (A), (B), (C), (D), or (E), as shown in Fig. 6, we have  $ \phi_T(Y)= \deg_T(v_1)-2,4, 3,3$, and 4, respectively.
Remark 4.3. The conditions (A), (B), (C), (D), (E) listed in Definition 4.2 are mutually exclusive. Case (A) is the only case where  $\operatorname{dist}_T(v_1,v_2)=0$. In cases (B), (C) and (D), we have
 $\deg_T(v_i)\geqslant 3$ for each
 $i\in [2]$, while in case (E), we have
 $\deg_T(v_2)=1$. Whether or not v 1 and v 2 are adjacent distinguishes (D) from (B) and (C). In case (B), it holds that
 $\deg_T(v_1)=\deg_T(v_2)=4$, whereas in case (C), we have
 $\deg_T(v_2)=3$.
Lemma 4.4. (Basic Lemma for score-2 split system)
Let  $k\geqslant 3$ be an integer, let T be a phylogenetic tree, and let
 $ Y \subseteq \mathrm{L}_T$. Then the following statements are equivalent:
(1) Y is a
$(k,2)$-set with respect to
$\mathcal{P}_{T,2}$.(2)
$k=\phi_T(Y)$ and (T, Y) is a 2-special configuration.


We refer to Lemma 4.4 as a basic lemma because it serves as a key step in connecting the graph structure with the split system structure. An analogous basic lemma for 2-split systems will be crucial for our work in [Reference Qian, Wu and Xie62]. To present a proof of Lemma 4.4, we require a convention and two additional technical lemmas.
Lemma 4.5. Let T be a phylogenetic tree, and let  $ Y\mid (\mathrm{L}_T\setminus Y) \in \mathcal{P}_{T,2}$. Assume that
 $ \{v_1u_1,v_2u_2\} = \partial_T(\mathrm{Ext}_{T,Y}) $, where
 $v_1,v_2\in \mathrm{Ext}_{T,Y}$. Then exactly one of the following holds:
(a)
$v_1=v_2$ and
$\deg_T(v_1)\geqslant 5$.(b)
$v_1v_2\in \mathrm{E}_T$ and
$\max\{\deg_T(v_1),\deg_T(v_2)\} \geqslant 4$.(c)
$T[\mathrm{Ext}_{T,Y}]$ is connected and
$\operatorname{dist}_T(v_1,v_2) \gt 1$.(d)
$T[\mathrm{Ext}_{T,Y}]$ is not connected, and either
$ u_1 \neq u_2 $ or
$ \deg_T(u_1) \geqslant 4 $.


Proof. Surely, exactly one of the following possibilities must occur: (a’)  $\operatorname{dist}_T(v_1, v_2)=0$; (b’)
 $\operatorname{dist}_T(v_1, v_2)=1$; (c’)
 $\operatorname{c}(T[\mathrm{Ext}_{T,Y}])=1$ while
 $\operatorname{dist}_T(v_1, v_2) \gt 1$; (d’)
 $\operatorname{c}(T[\mathrm{Ext}_{T,Y}]) \gt 1$, and hence
 $\operatorname{dist}_T(v_1, v_2) \gt 1$.
Case (c’) corresponds precisely to case (c).
Let  $\mathcal{U}=\{U\subseteq \mathrm{V}_T:\ U\mid W\in \widehat{\mathcal{S}}_{T,2}, Y=U\cap \mathrm{L}_T\}$. By definition,
 $\mathrm{Ext}_{T,Y}$ is the inclusion-minimal element in
 $\mathcal U$. This means that it cannot happen that
 $v_1v_2\in \mathrm{E}_T$ and
 $\deg_T(v_1)=\deg_T(v_2)=3$, as this would imply
 $\mathrm{Ext}_{T,Y}\setminus \{v_1,v_2\}\in \mathcal{U}$; see Fig. 7(A). We can also exclude the possibility of
 $v_1=v_2$ and
 $\deg_T(v_1)= 4$, as this would give
 $\mathrm{Ext}_{T,Y}-v_1\in \mathcal{U}$; see Fig. 7(B). Since
 $\mathbf{S}_{T,\{v_1u_1,v_2u_2\}} =
Y\mid (\mathrm{L}_T\setminus Y) \in \mathcal{P}_{T,2}$, Corollary 2.6 asserts that neither
 $v_1=v_2$ and
 $\deg_T(v_1)=3$ nor
 $u_1=u_2$ and
 $\deg_T(u_1)=3$ is valid. Therefore, we now find that cases (a’), (b’) and (d’) are equivalent to (a), (b) and (d), respectively.
Excluding two possibilities in the proof of Lemma 4.5. A)  $\widehat{\mathbf{S}}_{T,\{e_1,e_2\}}=U\mid W$,
 $\widehat{\mathbf{S}}_{T,\{e'_1,e'_2\}}=U'\mid W'$,
 $Y\subseteq U'\subseteq U'\cup \{v_1,v_2\}=U$. B)
 $\widehat{\mathbf{S}}_{T,\{e_1,e_2\}}=U\mid W$,
 $\widehat{\mathbf{S}}_{T,\{e'_1,e'_2\}}=U'\mid W'$,
 $Y\subseteq U'\subseteq U'\cup \{v_1\}=U$.

Convention 4.6
For the statements and proofs of Lemmas 4.4, 4.7 and Corollary 4.8, we introduce the following notations. Assume that T is a phylogenetic tree,  $Y\mid (\mathrm{L}_T\setminus Y)\in \mathcal{P}_{T,2}$, and
 $|{Y}|\geqslant 3$. Let
 $\partial_T(\mathrm{Ext}_{T,Y})=\{v_1u_1,v_2u_2\}$, where
 $\{v_1,v_2\}\subseteq \mathrm{Ext}_{T,Y}$ and
 $\deg_T(v_1)\geqslant \deg_T(v_2)$. Let
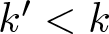
 $B_1,\ldots,B_{k'}$ be all distinct sets of the form
 $\mathrm{L}_T\cap \operatorname{C}_{T-v_1}[u]$, where
 $ u\in \operatorname{N}_T(v_1) \setminus \{u_1,u_2\}$ and
 $ v_2\notin \operatorname{C}_{T-v_1}[u] $; let
 $C_1,\ldots,C_{k^{\prime\prime}}$ be all distinct sets of the form
 $\mathrm{L}_T\cap \operatorname{C}_{T-v_2}[u]$, where
 $ u\in \operatorname{N}_T(v_2) \setminus \{u_1,u_2\}$ and
 $ v_1\notin \operatorname{C}_{T-v_2}[u] $. Let
 $B\doteq\bigcup_{i\in [k']}B_i$,
 $C\doteq\bigcup_{i\in [k^{\prime\prime}]}C_i$ and
 $D\doteq Y\setminus (B\cup C\cup \{v_1,v_2\})$. Note that
 $B\neq \emptyset$; B = C if and only if
 $v_1=v_2$;
 $C=\emptyset$ exactly when
 $\deg_T(v_2)=1$;
 $D=\emptyset$ exactly when
 $T[\mathrm{Ext}_{T,Y}]$ is not connected or
 $\operatorname{dist}_T(v_1,v_2)\leq 1$. See Fig. 8 for an illustration.
Distributions of Bi, Ci and D as described in Convention 4.6.

Lemma 4.7. Let T be a phylogenetic tree,  $Y\in \binom{\mathrm{L}_T}{\geqslant 3}$ and
 $Y\mid (\mathrm{L}_T\setminus Y)\in \mathcal{P}_{T,2}$. Then the following statements hold, where we use the convention in Convention 4.6.
(1) If
$v_1=v_2$ and
$\deg_T(v_1)\geqslant 5$, then
$\Gamma_{\mathcal{P}_{T,2}}(Y)=\{B_i\cup B_j:\ \{i,j\}\in \binom{[k']}{2}\}$.(2) If
$v_1v_2\in \mathrm{E}_T$ and
$ \deg_T(v_2)\geqslant 4$, then
$\Gamma_{\mathcal{P}_{T,2}}(Y)=\{B_i\cup C_j:\ i\in[k'], j\in [k^{\prime\prime}]\} \cup \{B,C\}$.(3) If
$v_1v_2\in \mathrm{E}_T$ and
$ \deg_T(v_1) \gt \deg_T(v_2)=3$, then
$\Gamma_{\mathcal{P}_{T,2}}(Y)=\{B_i\cup C:\ i\in [k']\} \cup \{B\}$.(4) If
$T[\mathrm{Ext}_{T,Y}]$ is connected and
$\operatorname{dist}_T(v_1,v_2) \gt 1$, then
$\Gamma_{\mathcal{P}_{T,2}}(Y)=\{B_i\cup C_j:\ i\in[k'], j\in [k^{\prime\prime}]\} \cup \{B\cup D, C\cup D\}$.(5) If
$\deg_T(v_2)=1$, then
\begin{equation*}\Gamma_{\mathcal{P}_{T,2}}(Y)=\begin{cases}
\{B_i+v_2:\ i\in [k']\} \cup \{B-x:\ x\in B\setminus \operatorname{N}_T(v_1)\}, &\text{if } \deg_T(v_1)=3,\\
\{B_i+v_2:\ i\in [k']\} \cup \{B-x:\ x\in B \}, &\text{if } \deg_T(v_1)\geqslant 4.
\end{cases} \end{equation*}(6) If
$\operatorname{c} (T[\mathrm{Ext}_{T,Y}]) \gt 1$ and
$\deg_T(v_2)\geqslant 3$, then
$\Gamma_{\mathcal{P}_{T,2}}(Y)=\{B_i\cup C:\ i\in [k']\} \cup \{B\cup C_i:\ i\in [k^{\prime\prime}]\}$.


Proof. Let  $V=\mathrm{V}_T$,
 $X=\mathrm{L}_T$ and
 $W=\mathrm{Ext}_{T,Y}$. Use the notation Δ for
 $\{Y'\subsetneq Y:\ Y' \mid(X\setminus Y')\in \mathcal{P}_{T,2}\}$. Note that
 $\Gamma_{\mathcal{P}_{T,2}}(Y)$ consists of all the inclusion-maximal elements of Δ. Let
 $Y'\in \Delta$ and
 $W'=\mathrm{Ext}_{T,Y'}$. Since T is a tree, deleting two edges from T results in exactly three connected components in the remaining graph. Therefore, we must have
 \begin{equation}
\{\operatorname{c}(T[W']),\operatorname{c}(T-W')\}=[2].
\end{equation}
CASE 1.  $T[W]$ is connected, and either
 $v_1\neq v_2$ or
 $\deg_T(v_1)\geqslant 5$. This includes cases (1), (2), (3) and (4).
Since  $T[W] $ is connected, both B and C are non-empty. This gives
 \begin{equation}
B\neq \emptyset, C\neq \emptyset, Y=B\cup C\cup D,
\end{equation}
and allows us to define  $ \mathcal{U}_1 \doteq \{B_i \cup C_j:\ i\in [k'],j\in [k^{\prime\prime}], B_i\neq C_j\}\subseteq 2^Y$. We claim that
 \begin{equation}
\mathcal{U}_1=\{Z\in \Gamma_{\mathcal{P}_{T,2}}(Y):\ Z\cap B\neq \emptyset, Z\cap C\neq \emptyset\}.
\end{equation}
Keeping in mind the validity of Eqs. (5) and (6), let us prove statements (1), (2), (3) and (4).
For statement (1), we are reduced to proving  $D=\emptyset$ and
 $\{B_i:\ i\in [k']\}=\{C_j:\ j\in [k^{\prime\prime}]\}$. These follow directly from
 $v_1=v_2$.
For statement (2), we only need to check that  $D=\emptyset$,
 $k',k^{\prime\prime}\geqslant 2$, and both B and C belong to Δ. The first and second conditions follow directly from
 $v_1v_2\in \mathrm{E}_T$ and
 $\deg_T(v_1)\geqslant \deg_T(v_2)\geqslant 4$, respectively. Because
 $\deg_T(v_1)\geqslant \deg_T(v_2)\geqslant 4$, by Corollary 2.6,
 $B\mid (X\setminus B)=\mathbf{S}_{T,\{v_1v_2,v_1u_1\}}\in \mathcal{P}_{T,2}$ and
 $C\mid (X\setminus C)=\mathbf{S}_{T,\{v_1v_2,v_2u_2\}}\in \mathcal{P}_{T,2}$, as desired.
To prove (3), it suffices to verify that  $D=\emptyset$,
 $k' \gt k^{\prime\prime}=1$ and
 $B \in \Delta$. The first two are direct from
 $v_1v_2\in \mathrm{E}_T$ and
 $\deg_T(v_1) \gt \deg_T(v_2)=3$. By Corollary 2.6, the last one follows from
 $\deg_T(v_1)\geqslant 4$ and
 $B\mid (X\setminus B)=\mathbf{S}_{T,\{v_1v_2,v_1u_1\}}$.
As for statement (4), it remains to show that  $D\neq \emptyset$ and that both
 $B\cup D$ and
 $C\cup D$ belong to Δ. The former follows directly from
 $\operatorname{c}(T[W])=1$ and
 $\operatorname{dist}_T(v_1,v_2) \gt 1$. To show the latter, by symmetry, it suffices to prove that
 $(B\cup D)\mid (X\setminus(B\cup D))\in \mathcal{P}_{T,2}$. According to Convention 4.6, there exists
 $w_2'\in \operatorname{N}_T(v_2)$ such that
 $D=X\cap \operatorname{C}_{T-v_1-v_2}[w_2']$. Note that
 $v_1,v_2,u_1$, and
 $w_2'$ are pairwise distinct. Then, by Corollary 2.6,
 $(B\cup D)\mid (X\setminus(B\cup D))=\mathbf{S}_{T,\{v_1u_1,v_2w_2'\}}\in \mathcal{P}_{T,2}$, as desired.
To complete the proof in this case, we need to verify Eq. (6). To obtain Eq. (6), we will deduce that  $\mathcal{U}_1 \subseteq \Delta$, and that
 \begin{equation}
Y'\subseteq B_i\cup C_j \end{equation}
whenever  $i\in [k']$ and
 $j\in [k^{\prime\prime}]$ are two elements satisfying
 $B_i\neq C_j$,
 $Y'\cap B_i\neq \emptyset$ and
 $Y'\cap C_j\neq \emptyset$.
Pick  $B_i\cup C_j\in \mathcal{U}_1$. On the one hand,
 $B_i\cup C_j\neq Y$. Otherwise, either
 $v_1=v_2$ and
 $\deg_T(v_1)=4$ or
 $v_1v_2\in \mathrm{E}_T$ and
 $\deg_T(v_1)=\deg_T(v_2)=3$, violating Lemma 4.5. On the other hand, by Convention 4.6, there are distinct
 $w_i\in \operatorname{N}_T(v_1)-v_2$ and
 $w_j\in \operatorname{N}_T(v_2)-v_1$ such that
 $B_i=X\cap \operatorname{C}_{T-v_1}[w_i]$ and
 $C_j=X\cap \operatorname{C}_{T-v_2}[w_j]$. As either
 $v_1\neq v_2$ or
 $\deg_T(v_1)\geqslant 5$, by Corollary 2.6,
 $(B_i\cup C_j) \mid (X\setminus (B_i \cup C_j))=\mathbf{S}_{T,\{v_1w_i,v_2w_j\}}$ belongs to
 $\mathcal{P}_{T,2}$, as desired. This proves
 $\mathcal{U}_1 \subseteq \Delta$.
If  $v_1,v_2\notin W'$, then, by Eq. (4),
 $\operatorname{c}(T[W']-\{v_1,v_2\})=\operatorname{c}(T[W'])\leq 2$. However,
 $Y'\setminus (B_i\cup C_j)$,
 $Y'\cap B_i$ and
 $Y'\cap C_j$ are pairwise non-reachable in
 $T[W']-\{v_1,v_2\}$, while
 $Y'\cap B_i\neq \emptyset$ and
 $Y'\cap C_j\neq \emptyset$. This forces Eq. (7) to hold. Henceforth, it remains to show that
 $v_1,v_2\notin W'$. Let us pick
 $x_0\in Y\setminus Y'$,
 $x_1\in X \cap \operatorname{C}_{T-v_1}[u_1]$ and
 $x_2\in X \cap \operatorname{C}_{T-v_2}[u_2]$. Then
 $x_0,x_1$, and x 2 are pairwise non-reachable leaves in
 $T-\{v_1,v_2\}$ and thus in
 $T-(W'\cup \{v_1,v_2\})$, which means
 $\operatorname{c}(T-(W'\cup \{v_1,v_2\})) \geqslant 3$. We thus derive from Eq. (4) that at least one of v 1 and v 2 does not belong to W′, say vt. As a result,
 $Y'\cap B_i\neq \emptyset$ and
 $Y'\cap C_j\neq \emptyset$ are non-reachable in
 $T[W']$. It must happen that
 $\operatorname{c}(T[W'])\geqslant 2$. This, together with Eq. (4), implies that
 $\operatorname{c}(T-W')=1$. As x 0 and
 $x_{3-t}$ are leaves of
 $T-W'$ that are non-reachable in
 $T-v_{3-t}$, we conclude that
 $v_{3-t} \notin W' $, thus completing our proof in Case 1.
CASE 2.  $ T [W] $ is not connected. This includes cases (5) and (6).
Before verifying statements (5) and (6), we establish two relevant facts. The first fact is that
 \begin{equation}
Y' \subseteq B_i \cup (Y\setminus B)
\end{equation}
holds for some  $i\in [k']$ whenever none of
 $B\setminus Y' $,
 $Y'\cap B $ and
 $Y'\setminus B $ is empty. Observe that, for distinct
 $i , j \in [k']$,
 $Y'\cap B_i$,
 $Y'\cap B_j$ and
 $Y'\setminus B $ are pairwise non-reachable in
 $T[W'-v_1]$. Henceforth, if
 $v_1\notin W'$, we can infer from
 $\operatorname{c}(T[W'-v_1])=\operatorname{c}(T[W'])\leq 2$ and
 $Y'\setminus B \neq \emptyset $ that Eq. (8) holds, as desired. Our task is thus to deduce
 $v_1\notin W'$. Choose
 $x_0\in B \setminus Y'$ arbitrarily. Since
 $\{x_0\}\cup (X\setminus Y)\subseteq X\setminus Y'=\mathrm{L}_{T-W'}$ and
 $v_1\in [\{x_0\}, X\setminus Y]_T$, we only need to check that
 $\operatorname{c}(T-W')=1$. By Lemma 4.5, it holds that either
 $ u_1 \neq u_2 $ or
 $ \deg_T(u_1) \geqslant 4 $. Hence there exists
 $\{w_1,w_2\}\in \binom{\operatorname{N}_T(u_1) \setminus \{v_1,v_2\}}{2}$. Pick
 $x_1\in X \cap \operatorname{C}_{T-u_1 }[w_1]$ and
 $x_2\in X\cap \operatorname{C}_{T-u_1 }[w_2]$. Observe that
 $x_0,x_1$, and x 2 are pairwise non-reachable in
 $T-u_1$ and thus in
 $T-W'-u_1$. Consequently,
 $\operatorname{c}(T-W'-u_1)\geqslant 3$. It then follows from
 $\operatorname{c}(T-W')\leq 2$ that
 $u_1\notin W'$. This, along with
 $Y'\cap B\neq \emptyset$ and
 $Y'\setminus B\neq \emptyset$, implies that
 $\operatorname{c}(T[W'])\geqslant 2$. We can thus apply Eq. (4) to obtain
 $\operatorname{c}(T-W')=1$, as desired.
We now want to deduce
 \begin{equation}
\mathcal{{U}}_2=\{Z\in \Gamma_{\mathcal{P}_{T,2}}(Y):\ Z\nsubseteq B, B\nsubseteq Z, Z\cap B\neq \emptyset\},
\end{equation}
where  $\mathcal{{U}}_2\doteq \{B_i\cup(Y\setminus B): i\in [k']\}$. If
 $\mathcal{{U}}_2 \subseteq \Delta$, then it is clear that Eq. (8) implies Eq. (9). So, what remains to prove is
 $\mathcal{{U}}_2 \subseteq \Delta$. As
 $T[W]$ is not connected, it holds that
 $k'=\deg_T(v_1)-1\geqslant 2$. Hence
 $Y\notin \mathcal{{U}}_2$. Let
 $Z=B_i\cup(Y\setminus B)$ for some
 $i\in [k']$. To finish the proof of
 $\mathcal{{U}}_2 \subseteq \Delta$, we aim to show that
 $Z\mid (X\setminus Z)\in \mathcal{P}_{T,2}$. Following Convention 4.6, there is a
 $w_i\in \operatorname{N}_T(v_1)-u_2$ such that
 $B_i=X\cap \operatorname{C}_{T-v_1}[w_i]$. By Corollary 2.6,
 $Z\mid (X\setminus Z)=\mathbf{S}_{T,\{v_1w_i,v_2u_2\}}\in \mathcal{P}_{T,2}$, as desired.
In the sequel, making use of the conditions  $k'\geqslant 2$ and Eq. (9) implicitly, we complete the proof of cases (5) and (6).
Let us start with statement (5). From  $\deg_T(v_2)=1$ it follows that
 $Y\setminus B=\{v_2\}$. Thus, for any set Z,
 $B\subsetneq Z \subseteq Y$ implies Z = Y; either B = Z or
 $Z\subseteq Y\setminus B$ implies
 $Z\mid (X\setminus Z)\notin \mathcal{P}_{T,2}$. These observations indicate that
 $\{Z\subseteq Y:\ B \subseteq Z \text{or } Z\cap B=\emptyset\}$ does not intersect with
 $\Gamma_{\mathcal{P}_{T,2}}(Y)$. Therefore, we only need to check that
 \begin{equation}
\{Z\in \Gamma_{\mathcal{P}_{T,2}}(Y):\ Z\subsetneq B\}=\begin{cases}
\{B-x:\ x\in B\setminus \operatorname{N}_T(v_1)\}, &\text{if } \deg_T(v_1)=3,\\
\{B-x:\ x\in B \}, &\text{if } \deg_T(v_1)\geqslant 4.
\end{cases}
\end{equation}
The proof of Eq. (10) is divided into two cases.
(1) Either
$\deg_T(v_1)\geqslant 4$ or
$B \cap \operatorname{N}_T(v_1)=\emptyset$.It is sufficient to verify that
$B-x\in \Delta$ for all
$x\in B$. Consider an arbitrary
$x\in B$, and let e be the edge incident to x in T. Whether
$\deg_T(v_1)\geqslant 4$ or
$B \cap \operatorname{N}_T(v_1)=\emptyset$, the edges
$v_1u_1$ and e cannot share a common endpoint of degree three in T. Consequently, by Corollary 2.6,
$(B-x)\mid (X\setminus(B-x))=\mathbf{S}_{T,\{v_1u_1,e\}}\in \mathcal{P}_{T,2}$, namely
$B-x\in \Delta$.(2)
$\deg_T(v_1)=3$ and
$B \cap \operatorname{N}_T(v_1)\neq \emptyset$.From
$\deg_T(v_1)=3$ we have
$|{B \cap \operatorname{N}_T(v_1)}|\leq 2$. If
$|{B \cap \operatorname{N}_T(v_1)}|= 2$, then
$|{Y}|=|{B}|+1=3$, and hence Eq. (10) follows from Corollary 2.7. Now, assume that
$B \cap \operatorname{N}_T(v_1)$ contains only one leaf x 0. Let
$\operatorname{N}_T(v_1)=\{u_1,x_0,w\}$. Then,
$(B-x_0)\mid (X\setminus(B-x_0))=\mathbf{S}_{T,\{v_1w\}}\notin \mathcal{P}_{T,2}$. Thus, a proper subset of B belonging to Δ must be a subset of B − x for some
$x\in B-x_0$. To show Eq. (10), it remains to verify that
$B-x\in \Delta$ for all
$x\in B-x_0$, which follows from similar arguments in the previous case.


It is time to prove statement (6). From  $\deg_T(v_2)\geqslant 3$ and
 $\operatorname{c}(T[W]) \gt 1$, it follows that
 $k^{\prime\prime}\geqslant 2$ and
 $C=Y\setminus B\neq \emptyset$. Since
 $C=Y\setminus B$, we obtain
 $\mathcal{U}_2= \{B_i\cup C:\ i\in [k']\}$. Let
 $ \mathcal{U}_2'\doteq \{C_j \cup B:\ j\in [k^{\prime\prime}]\}$. Our goal is to show that
 $ \Gamma_{\mathcal{P}_{T,2}}(Y)=\mathcal{U}_2\cup \mathcal{U}_2'$. By switching the roles of B and C and replacing
 $\{B_i:\ i\in [k']\}$ with
 $\{C_j:\ j\in[k^{\prime\prime}]\}$, we know from Eq. (9) that
 $\mathcal{U}_2' =\{Z\in \Gamma_{\mathcal{P}_{T,2}}(Y):\ Z\nsubseteq C, C\nsubseteq Z, Z\cap C\neq \emptyset\}$. Take
 $Z\in \Gamma_{\mathcal{P}_{T,2}}(Y)\setminus \mathcal{U}_2'$. Then
 $C\subsetneq Z \subsetneq Y$. This implies
 $Z\nsubseteq B$,
 $B\nsubseteq Z$, and
 $Z\cap B\neq \emptyset$. Thus ,
 $Z\in \mathcal{U}_2$ follows, as was to be shown.
For each family of sets  $\mathcal F$, designate by
 $\varrho_2(\mathcal{F})$ the set family
 $\{F\cap F':\ \{F,F'\}\in \binom{\mathcal{F}}{2}\}\setminus \{\emptyset\}$. For any k-partition π with
 $k\geqslant 3$, it is noteworthy that
 $\varrho_2(\operatorname{\mathcal{H}}_{\pi,2})=\pi$.
Proof of Lemma 4.4
Let  $V=\mathrm{V}_T$ and
 $X=\mathrm{L}_T$. When (1) holds, we necessarily have
 $|{Y}| \geqslant 3$ and
 $Y\mid(X\setminus Y)\in \mathcal{P}_{T,2}$. If (2) holds, the definition of a 2-special configuration implies
 $|{Y}| \geqslant 3$, and, in view of Corollary 2.6,
 $Y\mid(X\setminus Y)\in \mathcal{P}_{T,2}$. Henceforth, hereafter we shall assume that
 $|{Y}| \geqslant 3$,
 $Y\mid(X\setminus Y)\in \mathcal{P}_{T,2}$,
 $W\doteq \mathrm{Ext}_{T,Y}$, and adopt the convention from Convention 4.6 regarding
 $k',k^{\prime\prime},v_1,v_2,B,C,D$, etc.
Let  $\Pi\doteq \varrho_2(\Gamma_{\mathcal{P}_{T,2}}(Y))$. It is clear that condition (1) is equivalent to the following condition (1’):
(1’) Π is a k-partition of Y, and
$\Gamma_{\mathcal{P}_{T,2}}(Y)=\operatorname{\mathcal{H}}_{\Pi, 2}$.

According to Lemma 4.5, there are four cases to consider. We are going to establish the equivalence between (1’) ((1)) and (2) in each of these cases.
CASE 1.  $v_1=v_2$ and
 $\deg_T (v_1)\geqslant 5$, as given in Lemma 4.5 (a) and shown in Fig. 9(A).
In this case, (T, Y) is a 2-special configuration of type A and  $\phi_T(Y)=k'$. Hence, (2) amounts to requiring
 $k=k'$.
By Lemma 4.7 (1),  $ \Gamma_{\mathcal{P}_{T,2}}(Y) = \bigl\{B_i\cup B_j:\ \{i,j\}\in \binom{[k']}{2}\bigr\}$, which states that Y is a
 $(k',2)$-set with respect to
 $\mathcal{P}_{T,2}$. Therefore, (1) also holds if and only if
 $k=k' $.
CASE 2.  $v_1v_2\in \mathrm{E}_T$ and
 $\deg_T( v_1) =\max \{\deg_T( v_1), \deg_T( v_2) \}\geqslant 4$. This corresponds to Lemma 4.5 (b), as shown in Fig. 9(B).
In this case,  $D=\emptyset$,
 $k'=\deg_T (v_1)-2\geqslant 2$,
 $k^{\prime\prime}=\deg_T (v_2)-2$, and
 $ \phi_T(Y)=k'+k^{\prime\prime}$.
CASE 2.1.  $\deg_T (v_2)\geqslant 4$, which means that
 $k^{\prime\prime}\geqslant 2$.
In this case, (T, Y) is a 2-special configuration if and only if its type is B. Thus, (2) is equivalent to  $k'=k^{\prime\prime}=2$ and k = 4.
It follows from Lemma 4.7 (2) that
 \begin{equation*}
\Pi =\{B_i:\ i\in [k']\}\cup \{C_j:\ j\in [k^{\prime\prime}]\},
\end{equation*}
which is a  $(k'+k^{\prime\prime})$-partition of Y. Having a look into Lemma 4.7 (2) again, we find that
 $ \Gamma_{\mathcal{P}_{T,2}}(Y) =\operatorname{\mathcal{H}}_{\Pi,2} $ if and only if
 $k'=k^{\prime\prime}=2$. Combining these two facts yields that (1’) is also equivalent to
 $k'=k^{\prime\prime}=2$ and k = 4.
CASE 2.2.  $\deg_T (v_2)=3$, equivalently
 $k^{\prime\prime}=1$. In this case, (T, Y) is a 2-special configuration if and only if its type is C. Therefore, (2) is equivalent to
 $k=k'+1=3$.
In view of Lemma 4.7 (3), we have
 \begin{equation*}
\Pi =\{B_i:\ i\in [k']\}\cup \{C \},
\end{equation*}
which is a  $(k'+1)$-partition of Y. Comparing it with Lemma 4.7 (3), we know that
 $\Gamma_{\mathcal{P}_{T,2}}(Y) =\operatorname{\mathcal{H}}_{\Pi,2} $ if and only if
 $k'=2$. Thus, (1’) is also equivalent to
 $k=k'+1=3$.
CASE 3.  $T[W]$ is connected and
 $\operatorname{dist}_T(v_1,v_2) \gt 1$, as given in Lemma 4.5 (c) and shown in Fig. 9(C).
Different cases in the proof of Lemma 4.4. A) Case 1 B) Case 2 C) Case 3 D) Case 4

In this case,  $k'=\deg_T(v_1)-2\geqslant 1$,
 $k^{\prime\prime}=\deg_T(v_2)-2\geqslant 1$ and
 $\phi_T(Y)=k'+k^{\prime\prime}+1$. Additionally, (T, Y) is a 2-special configuration if and only if it is of type D, which is equivalent to
 $\deg_T(v_1)= \deg_T(v_2)=3 $. Hence, (2) holds if and only if
 $k'=k^{\prime\prime}=1$ and k = 3.
By Lemma 4.7 (4), it happens  $\Gamma_{\mathcal{P}_{T,2}}(Y)=\{B_i\cup C_j:\ i\in[k'], j\in [k^{\prime\prime}]\} \cup \{B\cup D, C\cup D\}$. Accordingly,
 \begin{equation*}
\Pi=\{B_i:\ i\in[k']\} \cup \{C_j:\ j\in [k^{\prime\prime}]\} \cup \{D\},
\end{equation*}
which is a  $(k'+k^{\prime\prime}+1)$-partition of Y. We see that
 $\Gamma_{\mathcal{P}_{T,2}}(Y)=\operatorname{\mathcal{H}}_{\Pi,2}$ if and only if
 $k'=k^{\prime\prime}=1$. Thus, (1’) is also equivalent to
 $k'=k^{\prime\prime}=1$ and
 $k=k'+k^{\prime\prime}+1=3$.
CASE 4.  $ T [W] $ is not connected, and either
 $u_1\neq u_2$ or
 $\deg_T(u_1)\geqslant 4$. This corresponds to the case of Lemma 4.5 (d), as illustrated in Fig. 9(D).
CASE 4.1.  $v_2\in \mathrm{L}_T$, namely
 $\deg_T(v_2)=1$.
Note that  $Y=B+v_2$. We thus derive from
 $|{Y}|\geqslant 3$ that
 $\phi_T(Y)=\deg_T(v_1)=k'+1\geqslant 3$.
CASE 4.1.1. Suppose  $\deg_T(v_1)=3 $, and hence (T, Y) is not a 2-special configuration and
 $k'=2$. In this case, statement (2) cannot hold. By virtue of
 $k'=2$, Lemma 4.7 (5) yields that
 $\{B_i+v_2:\ i\in [2]\}\subseteq \Gamma_{\mathcal{P}_{T,2}}(Y)$ and
 $\{v_2\}\in \Pi$. Thus, if
 $\Gamma_{\mathcal{P}_{T,2}}(Y)=\operatorname{\mathcal{H}}_{\Pi,2}$, then
 $\Pi=\bigl\{\{v_2\}, B_1, B_2 \bigr\} $ and hence
 $B=B_1\cup B_2 \in \operatorname{\mathcal{H}}_{\Pi,2} \setminus \Gamma_{\mathcal{P}_{T,2}}(Y)$. Therefore, statement (1’) cannot hold either.
CASE 4.1.2. Suppose  $\deg_T(v_1)\geqslant 4$. Whenever (T, Y) is a 2-special configuration, its type must be E. By further taking into account that
 $|{Y}|=|{B}|+1\geqslant k'+1=\phi_T(Y)=\deg_T(v_1)\geqslant 4$, (2) holds if and only if
 $k' = |{B}| =3 $.
From Lemma 4.7 (5) and  $|{B}|\geqslant 3$, it follows that
 \begin{equation*}
\Pi=\binom{B}{|{B}|-2} \cup \left(\bigcup_{i: |{B_i}|\geqslant 2, i\in [k']}\binom{B_i}{|{B_i}|-1}\right) \cup \{B_i:\ i\in [k']\} \cup \left\{\{v_2\}\right\}.
\end{equation*}
As  $\binom{B}{|{B}|-2}\subseteq \Pi$, Π is a k-partition for
 $k\geqslant 3$ only if
 $|{B}|=3$. If
 $|{B}|=3$, then
 $k'=3$ and by Lemma 4.7 (5) we see that (1’) holds. Thus (1’) is also equivalent to
 $k' = |{B}| =3 $.
CASE 4.2.  $\deg_T(v_2)\geqslant 3$.
In this case,  $ k'=\deg_T(v_1)-1\geqslant 2$,
 $k^{\prime\prime}= \deg_T(v_2)-1\geqslant 2$ and (2) cannot hold. By Lemma 4.7 (6),
 $B_i\cup C_j\in \Pi$ for each
 $i\in [k']$ and
 $j\in [k^{\prime\prime}]$. Thus, Π is not a partition, implying that (1’) cannot hold either.
Corollary 4.8. Let T be a phylogenetic tree and let  $Y\subseteq \mathrm{L}_T$. Suppose (T, Y) is a 2-special configuration and
 $\varrho_2(\Gamma_{\mathcal{P}_{T,2}}(Y))=\{Y_1, \dots, Y_k \}\in \binom{2^Y}{k}$. Then the connected components of
 $T[\mathrm{Ext}_{T,Y}]-(\{v_1,v_2\}\setminus \mathrm{L}_T)$ can be enumerated as
 $V_1,\ldots,V_k$ such that
 $Y_i=V_i\cap \mathrm{L}_T$ for all
 $i\in [k]$.
Proof. As (T, Y) is a 2-special configuration and  $\varrho_2(\Gamma_{\mathcal{P}_{T,2}}(Y))=\{Y_1, \dots, Y_k \}$, from Lemma 4.4 it follows that Y is a
 $(k,2)$-set with respect to
 $\mathcal{P}_{T,2}$ and
 $k=\phi_T(Y)=\operatorname{c}(T[\mathrm{Ext}_{T,Y}]-(\{v_1,v_2\}\setminus \mathrm{L}_T))$. Thus we can enumerate the connected components of
 $T[\mathrm{Ext}_{T,Y}]-(\{v_1,v_2\}\setminus \mathrm{L}_T)$ as
 $V_1,\ldots,V_k$.
Adopt notations from Convention 4.6. We see from Fig. 6 that
 \begin{equation*}\{V_i\cap \mathrm{L}_T: i\in [k]\}=\begin{cases}
\{B_i: i\in [k']\}\cup \{C_j:\ j\in [k^{\prime\prime}]\}, & \text{if} \ (T,Y) \ \text{is of type } \mathtt{A}, \mathtt{B} \text{ or } \mathtt{C},\\
\{B, C, D\}, & \text{if} \ (T,Y) \ \text{is of type } \mathtt{D},\\
\bigl\{\{y\}:\ y\in Y \bigr\}, & \text{if} \ (T,Y) \ \text{is of type } \mathtt{E}.
\end{cases}\end{equation*}
According to Lemma 4.7, we have
 \begin{equation*}\varrho_2(\Gamma_{\mathcal{P}_{T,2}}(Y))=\begin{cases}
\{B_i: i\in [k']\}\cup \{C_j:\ j\in [k^{\prime\prime}]\}, & \text{if} \ (T,Y) \ \text{is of type } \mathtt{A}, \mathtt{B} \text{ or } \mathtt{C},\\
\{B, C, D\}, & \text{if} \ (T,Y) \ \text{is of type } \mathtt{D},\\
\bigl\{\{y\}:\ y\in Y \bigr\}, & \text{if} \ (T,Y) \ \text{is of type } \mathtt{E}.
\end{cases}\end{equation*}
Therefore, it follows that  $\{V_i\cap \mathrm{L}_T:\ i\in [k]\}=\varrho_2(\Gamma_{\mathcal{P}_{T,2}}(Y))=\{Y_1, \dots, Y_k \}$.
Remark 4.9. Let T be a phylogenetic tree and let  $Y\subseteq \mathrm{L}_T$ be a
 $(k,2)$-set with respect to
 $\mathcal{P}_{T,2}$. Suppose
 $\varrho_2(\Gamma_{\mathcal{P}_{T,2}}(Y))=\{Y_1,\ldots,Y_k\}$,
 $\partial_T(\mathrm{Ext}_{T,Y})=\{v_1u_1,v_2u_2\}$,
 $\{v_1,v_2\}\subseteq \mathrm{Ext}_{T,Y}$ and
 $\deg_T(v_1)\geqslant \deg_T(v_2)$. By Lemma 4.4, (T, Y) is a 2-special configuration.
(1) If (T, Y) is of type B or C, then by Corollary 4.8, we can let
$\{Y_1,Y_2\}=\{\mathrm{L}_T\cap \operatorname{C}_{T-\{v_1,v_2\}}[v]:\ v\in \operatorname{N}_T(v_1)-u_1\}$ and
$\{Y_3,\ldots,Y_k\}=\{\mathrm{L}_T\cap \operatorname{C}_{T-\{v_1,v_2\}}[v]:\ v\in \operatorname{N}_T(v_2)-u_2\}$. See Figs. 6(B) and 6(C).(2) If (T, Y) is of type D, then by Corollary 4.8, we can let
$\{Y_1,Y_2\}=\{\mathrm{L}_T\cap \operatorname{C}_{T-\{v_1,v_2\}}[v]:\ v\in \operatorname{N}_T(v_1)-u_1\}$ and
$\{Y_2,Y_3\}=\{\mathrm{L}_T\cap \operatorname{C}_{T-\{v_1,v_2\}}[v]:\ v\in \operatorname{N}_T(v_2)-u_2\}$. See Fig. 6(D).(3) If (T, Y) is of type E, then we can let
$Y_1\cup Y_2\cup Y_3=\mathrm{L}_T\cap \operatorname{N}_T(v_1)$ and
$Y_4=\{v_2\}$. For distinct
$i,j\in [4]$, let
$Y_{ij}=\mathrm{L}_T\setminus (Y_i\cup Y_j)$. See Fig. 6(E).(4) If the type of (T, Y) is one of A, B, C and D, then let
$Y_{k+1}=\mathrm{L}_T\cap \operatorname{C}_{T-v_1}[u_1]$ and
$Y_{k+2}=\mathrm{L}_T\cap \operatorname{C}_{T-v_2}[u_2]$. For distinct
$i,j\in [k+2]$, let
$Y_{ij}=\mathrm{L}_T\setminus (Y_i\cup Y_j)$. See Figs. 6(A), 6(B), 6(C) and 6(D).


Corollary 4.10. Let T be a phylogenetic tree, and let  $Y\subseteq \mathrm{L}_T$. Suppose (T, Y) is a 2-special configuration whose type is not E, and adopt the notations from Remark 4.9. Then the following two statements hold for all
 $\{i,j\}\in \binom{[k+2]}{2}$.
(1) If
$v_1,v_2\in [Y_i,Y_j]_T$, then Yij is a
$(k,2)$-set with respect to
$\mathcal{P}_{T,2}$.(2) If the type of (T, Y) is A, then
$ \varrho_2(\Gamma_{\mathcal{P}_{T,2}}(Y_{ij})) = \{Y_p:\ p\in [k+2]\setminus \{i,j\}\} $.


Proof. (1). By Corollary 4.8 and Remark 4.9, there exist  $w_1, w_2\in \operatorname{N}_T(v_1)\cup \operatorname{N}_T(v_2)$ such that
 $Y_i=\mathrm{L}_T \cap \operatorname{C}_{T-\{v_1,v_2\}}[w_1]$ and
 $Y_j=\mathrm{L}_T \cap \operatorname{C}_{T-\{v_1,v_2\}}[w_2]$. Since
 $v_1,v_2\in [Y_i,Y_j]_T$, it follows that
 $v_1,v_2\in [w_1,w_2]_T$. Thus, by symmetry we may assume that
 $w_1\in \operatorname{N}_T(v_1)$ and
 $w_2\in \operatorname{N}_T(v_2)$. Denote
 $\operatorname{C}_{T-\{w_1,w_2\}}[v_1]$ by W. Then
 $Y_{ij}=W\cap \mathrm{L}_T$,
 $\partial_T(W)= \{v_1w_1,v_2w_2\}$ and
 $\{v_1,v_2\} \subseteq W$. As v 1 and v 2 satisfy Eq. (2), by Lemma 2.11, W is exactly
 $\mathrm{Ext}_{T,Y_{ij}}$. Because
 $T[W]$ is connected, by the definitions of types A, B, C and D,
 $(T,Y_{ij})$ is a 2-special configuration of the same type as (T, Y). Then, by Lemma 4.4, Yij is a
 $(k,2)$-set with respect to
 $\mathcal{P}_{T,2}$, as desired.
(2). From the above proof of (1), we know that  $(T, Y_{ij})$ is a 2-special configuration of type A. Since
 $v_1=v_2$ and
 $Y_{ij}\mid (Y_i\cup Y_j)=\mathbf{S}_{T,\{v_1w_1,v_2w_2\}}$, the claim follows directly from Corollary 4.8.
4.2. Type A and type E
We begin with a definition of certain structures associated with a split system. It will soon become evident that these structures are designed to encode 2-special configurations of type A and type E.
Definition 4.11. Let  $\mathcal{S}$ be a split system on a finite set X and let
 $k\geqslant 3$ be an integer. We use
 $\mathcal{Y}_k(\mathcal{S})$ to denote the set family consisting of all
 $(k,2)$-sets with respect to
 $\mathcal{S}$. Let
 $\mathcal{Y}_k^{\mathtt{A}}(\mathcal{S})$ consist of all
 $Y\in \mathcal{Y}_k(\mathcal{S})$ such that
 $X\setminus (Y_i \cup Y_j)\in \mathcal{Y}_k(\mathcal{S})$ for all distinct
 $i,j\in [k]$, where
 $\{Y_1,\ldots, Y_k\}= \varrho_2(\Gamma_{\mathcal{S}}(Y))$. Let
 $\mathcal{Y}^{\mathtt{A}}(\mathcal{S})=\bigcup_{i\geqslant 3}\mathcal{Y}_i^{\mathtt{A}}(\mathcal{S})$. Let
 $\mathcal{Y}^{\text{claw}}(\mathcal{S})$ consist of all
 $\{x,y,z\}\in \binom{X}{3}$ for which there exists
 $\{w_1,w_2,w_3\}\in \binom{X\setminus \{x,y,z\}}{3}$ such that
 $\{x,y,z,w_i\}\in \mathcal{Y}_4(\mathcal{S})$ for all
 $i\in [3]$.
Let T be a phylogenetic tree, and let  $k\geqslant 5$. It follows directly from Lemma 4.4 that
 $Y\in \mathcal{Y}_k^{\mathtt{A}}(\mathcal{P}_{T,2})$ only if (T, Y) is a 2-special configuration of type A. However, a stronger version of this statement is required, which we establish in Lemma 4.13.
Lemma 4.12. Let T be a phylogenetic tree and let  $Y\subseteq \mathrm{L}_T$ be a
 $(k,2)$-set with respect to
 $\mathcal{P}_{T,2}$. Adopt the convention in Remark 4.9.
(1) Suppose the type of (T, Y) is B. If both Y 12 and Y 34 are
$(4,2)$-sets with respect to
$\mathcal{P}_{T,2}$, then
$T\cong \widetilde{\mathtt{A}}_0$.(2) If the type of (T, Y) is C or D, then Y 12 is not a
$(3,2)$-set with respect to
$\mathcal{P}_{T,2}$.(3) Suppose the type of (T, Y) is E. For any
$\{i,j\}\in \binom{[3]}{2}$, Yij is a
$(4,2)$-set with respect to
$\mathcal{P}_{T,2}$ if and only if
$T\cong \widetilde{\mathtt{A}}_0$.


Proof. We start with (1). By Lemma 4.4, Y 12 being a  $(4,2)$-set with respect to
 $\mathcal{P}_{T,2}$ implies that (T, Y) is a 2-special configuration. Clearly,
 $Y_{12}=\mathbf{S}_{T,\{v_1u_1,v_1v_2\}}$ while u 1 and v 2 satisfy Eq. (2). Thus, by Lemma 2.11,
 $\mathrm{Ext}_{T,Y_{12}}=\operatorname{C}_{T-v_1}[u_1]\cup \operatorname{C}_{T-v_1}[v_2]$. Since
 $T[\mathrm{Ext}_{T,Y_{12}}]$ is not connected, the only possible type of
 $(T,Y_{12})$ is E. The definition of type E requires that each Yi,
 $i\in \{3,4,5,6\}$, consists of a single element. Similarly, if Y 34 is a
 $(4,2)$-set with respect to
 $\mathcal{P}_{T,2}$, then all Yi,
 $i\in \{1,2,5,6\}$, have size one. In conclusion, if both Y 12 and Y 34 are
 $(4,2)$-sets with respect to
 $\mathcal{P}_{T,2}$, then all Yi,
 $i\in [6]$, are singleton sets, which implies that
 $T\cong \widetilde{\mathtt{A}}_0$.
Now, we consider (2). Suppose the type of (T, Y) is C or D. Let w 2 be the unique vertex in  $\operatorname{N}_T(v_2)\cap [v_1,v_2]_T$. Then
 $Y_{12}=\mathbf{S}_{T,\{v_1u_1, w_2v_2\}}$ while u 1 and v 2 satisfy Eq. (2). Hence, by Lemma 2.11,
 $\mathrm{Ext}_{T,Y_{12}}=\operatorname{C}_{T-v_1}[u_1]\cup \operatorname{C}_{T-w_2}[v_2]$. Note that
 $T[\mathrm{Ext}_{T,Y_{12}}]$ is not connected and
 $\deg_T(v_2)=3$. By definition, (T, Y) is not a 2-special configuration. Consequently, by Lemma 4.4, Y 12 is not a
 $(3,2)$-set with respect to
 $\mathcal{P}_{T,2}$.
At last, we examine (3). By symmetry, suppose  $\{i,j\}=[2]$. Denote the only leaf in Yi by yi for each
 $i\in [3]$. It is clear that
 $Y_{12}\mid \{y_1,y_2\}=\mathbf{S}_{T,\{v_1y_3,v_1u_1\}}$. Let
 $U\doteq \mathrm{V}_T\setminus \{y_1,y_2,v_1\}$. From
 $\widehat{\mathbf{S}}_{T,\{v_1y_3,v_1u_1\}}=U\mid \{y_1,y_2,v_1\}$, it follows that
 $\{y_3,v_2\}\subseteq\mathrm{Ext}_{T,Y_{12}}\subseteq U$. Since y 3 and v 2 are not reachable in
 $T[U]$,
 $T[\mathrm{Ext}_{T,Y_{12}}]$ is not connected. Therefore, by Lemma 4.4, Y 12 is a
 $(4,2)$-set with respect to
 $\mathcal{P}_{T,2}$ if and only if
 $(T,Y_{12})$ is a 2-special configuration of type E. The latter condition is equivalent to
 $\mathrm{L}_T\setminus \{y_1,y_2,y_3\}$ being a claw of T, i.e.,
 $T\cong \widetilde{\mathtt{A}}_0$.
Lemma 4.13. Let T be a phylogenetic tree with  $T\ncong \widetilde{\mathtt{A}}_0$. For any
 $Y\subseteq \mathrm{L}_T$, we have
 $Y\in \mathcal{Y}^{\mathtt{A}}(\mathcal{P}_{T,2})$ if and only if (T, Y) is a 2-special configuration of type A.
Proof. The sufficiency follows from Corollary 4.10 (1), while the necessity follows from Lemma 4.12.
We proceed to investigate how to encode the possible claw structure of a tree based on its score-2 split system.
Lemma 4.14. Let T be a phylogenetic tree, and let  $Y\subseteq \mathrm{L}_T$ be a
 $(4,2)$-set with respect to
 $\mathcal{P}_{T,2}$. Suppose the type of (T, Y) is B and adopt the notations in Remark 4.9. Let
 $j\in \{5,6\}$. If there exists a set
 $I\in \binom{[4]}{3}$ and a vertex
 $w\in Y_j$ such that
 $((\bigcup_{i\in I}Y_i)+w)\mid ((\bigcup_{i\in [6]\setminus I}Y_i)-w)\in \mathcal{P}_{T,2}$, then
 $Y_j=\{w\}$.
Proof. By symmetry, it suffices to verify the result for  $I=[3]$ and
 $j\in \{5,6\}$. We only consider the case
 $I=[3]$ and j = 5, as the case
 $I=[3]$ and j = 6 can be verified with the same argument.
There exist  $e_1,e_2\in \mathrm{E}_T$ such that
 $((\bigcup_{i\in [3]}Y_i)+w)\mid ((\bigcup_{i\in \{4,5,6\}}Y_i)-w)=\mathbf{S}_{T,\{e_1,e_2\}}$. Let
 $T'=T-V_5$ and
 $w_4\in V_4\cap \operatorname{N}_T(v_2)$, where
 $V_i\doteq \operatorname{C}_{T-\{v_1,v_2\}}[Y_i]$ for
 $i=4,5$. Because
 $v_2w_4$ and
 $v_2u_2$ are not incident with a common vertex of degree 3 in T′, combining Lemma 2.8 and Corollary 2.6 yields
 $\mathbf{S}_{T',\{e_1,e_2\}\cap \mathrm{E}_{T'}}=\mathbf{S}_{T,\{e_1,e_2\}}|_{\mathrm{L}_{T'}}=(Y_1\cup Y_2\cup Y_3)\mid (Y_4 \cup Y_6)=\mathbf{S}_{T',\{v_2w_4,v_2u_2\}}\in \mathcal{P}_{T',2}$. This implies
 $e_1,e_2\in \mathrm{E}_{T'}$. Consequently,
 $\mathbf{S}_{T,\{e_1,e_2\}}|_{Y_5}=\{w\}\mid (Y_5-w)$ is improper, which means
 $Y_5=\{w\}$, as desired.
Lemma 4.15. Let T be a phylogenetic tree with at least seven leaves. Suppose  $\max_{v\in \mathrm{V}_T}\deg_T(v)\leq 4$. For any
 $\{x, y,z \}\in \binom{\mathrm{L}_T}{3}$,
 $\{x,y,z\}\in \mathcal{Y}^{\text{claw}}(\mathcal{P}_{T,2}) $ if and only if
 $\{x,y,z\}$ is a claw of T.
Proof. We assume that  $\{x,y,z\}$ is a claw of T. Let u 0 be the common neighbor of
 $x,y$, and z in T, and let v 0 be the only vertex in
 $ \operatorname{N}_T(u_0)\setminus\{x,y,z\}$. Let
 \begin{equation*}W=\begin{cases}
\mathrm{L}_T\setminus (\operatorname{N}_T(v_0)\cup \{x,y,z\}), & \text{if }\deg_T(v_0)=3,\\
\mathrm{L}_T\setminus \{x,y,z\} ,& \text{otherwise}.
\end{cases}\end{equation*}
It follows from  $|{\mathrm{L}_T}|\geqslant 7$ that
 $|{W}|\geqslant 3$. Let
 $w\in W$. It is easy to verify that
 $\mathrm{Ext}_{T,\{x,y,z,w\}}=\{x,y,z,w,u_0\}$, and thus
 $(T,\{x,y,z,w\})$ is a 2-special configuration of type E. Then, by Lemma 4.4,
 $\{x,y,z,w\}$ is a
 $(4,2)$-set with respect to
 $\mathcal{P}_{T,2}$. Consequently,
 $\{x,y,z\}\in \mathcal{Y}^{\text{claw}}(\mathcal{P}_{T,2}) $.
Conversely, suppose that  $\{x,y,z\}\in \mathcal{Y}^{\text{claw}}(\mathcal{P}_{T,2}) $. That is, there exists
 $\{w_1, w_2, w_3\}\in \binom{\mathrm{L}_T\setminus \{x,y,z\}}{3}$ such that
 $\{x,y,z,w_i\}$ is a
 $(4,2)$-set with respect to
 $\mathcal{P}_{T,2}$ for all
 $i\in [3]$. This, together with Lemma 4.4 and the condition
 $\max_{v\in \mathrm{V}_T}\deg_T(v)\leq 4$, reveals that
 $(T,\{x,y,z,w_i\})$ is a 2-special configuration of type B or E for each
 $i\in[3]$. Since a leaf is contained in at most one claw of T, to prove that
 $\{x,y,z\}$ is a claw of T, it suffices to show that the type of
 $(T, \{x,y,z,w_i\})$ is E for each
 $i\in [3]$, which would mean that
 $\{x,y,z,w_i\}$ contains a claw of T. If
 $(T,\{x,y,z,w_i\})$ is of type B, then applying Lemma 4.14 with
 $Y=\{x,y,z,w_i\}$ yields
 $\mathrm{L}_T\setminus Y=\{w_1, w_2 , w_3\}-w_i$, which violates the assumption
 $|{\mathrm{L}_T}|\geqslant 7$; see Fig. 10.
A possible tree appeared in the proof of Lemma 4.15.

5. Tree reconstruction algorithm
Let us present Algorithm 2, our algorithm for recovering a phylogenetic tree from its score-2 split system. After demonstrating in Lemma 5.2 how Algorithm 2 accomplishes the three reduction steps mentioned in  $\S$ 1, we will prove Theorem 1.3.
Lemma 5.1. Let T be a phylogenetic X-tree. Then,  $T\in \{\mathtt{A}_0, \widetilde {\mathtt{A}}_0 \}$ if and only if
 $|X|=6$ and
 $\mathcal{P}_{T,2}=\{Y\mid (X\setminus Y):\ Y\in \binom{X}{2}\}$.
Proof. Suppose  $T\in \{\mathtt{A}_0, \widetilde{\mathtt{A}}_0\}$. It is straightforward to verify that
 $|X|=6$ and
 $\mathcal{S}_{T,2}=\{Y\mid(X\setminus Y): \ Y\in \binom{X}{2} \}$. Since T has no vertex of degree 3, it follows from Remark 2.4 and Corollary 2.6 that
 $\mathcal{P}_{T,2}=\mathcal{S}_{T,2}$.
Conversely, suppose  $|X|=6$ and
 $\mathcal{P}_{T,2}=\{Y\mid(X\setminus Y): Y\subseteq X, |{Y}|=2\}$. Let us pick
 $u,v\in \mathrm{V}_T\setminus X$ such that
 $\operatorname{dist}_T(u,v)=\max\{\operatorname{dist}_T(w,w'):\ w,w'\in \mathrm{V}_T\setminus X\}$. Then we must have
 $|{\operatorname{N}_T(u)\setminus X}|\leq 1$ and
 $
|{\operatorname{N}_T(v)\setminus X}|\leq 1$. We know from Corollary 2.7 that T contains no cherry. Consequently,
 $|{\operatorname{N}_T(u)\cap X}|\geqslant 3$ and
 $|{\operatorname{N}_T(v)\cap X}|\geqslant 3$. Notice that
 $|X|=6$. We thus conclude that
 $T\cong \mathtt{A}_0$ if u = v, and
 $T\cong \widetilde{\mathtt{A}}_0$ if u ≠ v.
Lemma 5.2. Let X be a finite set with  $ |X| \geqslant 2 $, and let
 $ \mathcal{S} $ be a split system on X.
(1) If
$ \mathcal{S} \ncong \mathcal{P}_{\mathtt{A}_0,2} $, then Algorithm 2 outputs either a singleton set or the empty set.(2) The output of Algorithm 2 is the set of all phylogenetic X-trees T with
$ \mathcal{P}_{T,2} = \mathcal{S} $ up to X-isomorphism.


Proof. According to Lemma 5.1,  $ \mathcal{S} $ is isomorphic to
 $ \mathcal{P}_{\mathtt{A}_0,2} $ if and only if
 $|X|=6$ and
 $\mathcal{S} = \{Y\mid (X\setminus Y):\ Y\subseteq X, |{Y}|=2 \}$. Except for its Line 7, Algorithm 2 always returns either a singleton set or the empty set. We thus verify (1).
Suppose there is a phylogenetic X-tree T such that  $\mathcal{S}=\mathcal{P}_{T,2}$. To prove (2), we need to show that, up to X-isomorphism, T is a member of the output of Algorithm 2.
If  $ |X| = 2 $, the only phylogenetic X-tree is the tree with one edge, whose score-2 split system is
 $\emptyset$. Lines 1 to 5 of Algorithm 2 handle this case. If
 $ \mathcal{S} \cong \mathcal{P}_{\mathtt{A}_0,2} $, then, by Lemma 5.1, the phylogenetic X-trees output in Line 7 are exactly all phylogenetic X-trees whose score-2 split systems are
 $\mathcal{S}$. In the remainder of this proof, assume
 $|X|\geqslant 3$ and
 $\mathcal{S}\ncong \mathcal{P}_{\mathtt{A}_0,2}$. Hence, T is not isomorphic to
 $ \widetilde{\mathtt{A}}_0 $.
CASE 1.  $\mathcal{Y}^{\mathtt{A}}(\mathcal{S})\neq \emptyset$. Lines 9 to 19 of Algorithm 2 address this case.
Select a Y from  $\mathcal{Y}^{\mathtt{A}}(\mathcal{S})$ as described in Line 10. By Lemma 4.13, (T, Y) is a 2-special configuration of type A. This implies the existence of a
 $v_1\in \mathrm{Ext}_{T,Y}$ that serves as an endpoint of both edges in
 $\partial_T(\mathrm{Ext}_{T,Y})$. By Corollary 4.8 and Corollary 4.10 (2), the set
 $\{Y_1,\ldots,Y_{k+2}\}$ defined in Lines 11 and 12 corresponds precisely to
 $\{X\cap \operatorname{C}_{T-v_1}[u]:\ u\in \operatorname{N}_T(v_1)\}$. Subsequently, by Lemma 3.3, Algorithm 1 offers a method to reconstruct T from
 $ \mathcal{P}_{T,2} $ and
 $ Y_1 \mid \dots \mid Y_{k+2} $. In this case, Algorithm 2 outputs
 $ \{T\} $, as demonstrated in its Lines 13 and 15.
CASE 2.  $\mathcal{Y}^{\mathtt{A}}(\mathcal{S})= \emptyset$.
Execute the while loop in Lines 23 to 28. Suppose the while loop terminates after m iterations. For each  $k\in [m]$, the values of variables
 $\{x,y\}$, X,
 $\mathcal{S}'$ and
 $\mathcal{P}^\text{cherry}$ in Lines 24 to 27 at the end of the k-th iteration are represented as
 $\{x_k,y_k\}$, Xk,
 $\mathcal{S}_k$ and
 $\mathcal{P}^\text{cherry}_k$, respectively. Let
 $T_0=T$,
 $X_0=X$,
 $\mathcal{S}_0=\mathcal{S}=\mathcal{P}_{T,2}$ and
 $\mathcal{P}^\text{cherry}_0$ be the set defined in Line 22.
We claim that, for each  $k\in [m]$,
 $\mathcal{S}_k$ is the score-2 split system on a phylogenetic Xk-tree
 $T_k\doteq T_{k-1}-\{x_k,y_k\}$, where
 $\{x_k,y_k\}$ is a cherry of
 $T_{k-1}$. Since
 $\mathcal{S}_0=\mathcal{P}_{T_0,2}$, we only need to prove the claim inductively for each
 $k\in [m]$ under the hypothesis that
 $\mathcal{S}_{k-1}=\mathcal{P}_{T_{k-1},2}$ for a phylogenetic
 $X_{k-1}$-tree
 $T_{k-1}$. By virtue of Corollary 2.7,
 $\{x_k,y_k\}\in \mathcal{P}^\text{cherry}_{k-1}$ is a cherry of
 $T_{k-1}$; and then by Lemma 3.1, the split system
 $\mathcal{S}_k$ is exactly the score-2 split system on the phylogenetic Xk-tree
 $T_k= T_{k-1}-\{x_k,y_k\}$. Our claim thus follows. We shall repeatedly use this claim implicitly in our remaining proof.
For each  $k\in [m]$,
 $ T_{k-1} $ is obtained from Tk by adding two edges
 $ x_kv_{\{x_k,y_k\}} $ and
 $ y_kv_{\{x_k,y_k\}}$, where
 $v_{\{x_k,y_k\}}$ is defined in Line 25. So, we can construct T from Tm step by step, as demonstrated in Lines 40 to 44. Our task now reduces to finding Tm from the Xm-split system
 $ \mathcal{S}_m $.
Observe that  $\mathcal{S}_m \ncong \mathcal{P}_{\mathtt{A}_0,2}$, which also means
 $T_m \ncong \widetilde{\mathtt{A}}_0$. Otherwise, due to
 $\mathcal{S} \ncong \mathcal{P}_{\mathtt{A}_0,2}$, the integer m must be positive and
 $T_{m-1}-\{x_m,y_m\}=T_m \cong \widetilde{\mathtt{A}}_0$. The latter means
 $|{X_{m-1}}|=7$ and
 $T_{m-1}$ contains exactly one cherry. From Corollary 2.7 and
 $\mathcal{S}_{m-1}=\mathcal{P}_{T_{m-1},2}$, we have
 $|{\mathcal{P}^\text{cherry}_{m-1}}|=1$. Thus, the while loop terminates after m − 1 iterations, contradicting our supposition.
It follows from Lemma 4.13 and  $\mathcal{Y}^{\mathtt{A}}(\mathcal{S})= \emptyset$ that
 $\max_{v \in \mathrm{V}_T} \deg_T(v) \leq 4 $. As Tm is a subtree of T, it also holds that
 $\max_{v \in \mathrm{V}_{T_m}} \deg_{T_m}(v) \leq 4 $. Because the while loop in Lines 23 to 28 terminates, there are three cases:
 $ |{X_m}| =3$;
 $ \mathcal{P}^\text{cherry}_m = \emptyset $;
 $ |{X_m}| = 7 $ and
 $ |{\mathcal{P}^\text{cherry}_m}| \leq 1$.
CASE 2.1.  $ 3 \leq |{X_m}| \leq 6 $. Lines 29 to 30 of Algorithm 2 deal with this case.
If  $|{X_m}| = 3$, we must have
 $T_m \cong \mathrm{K}_{1,3}$.
When  $4\leq |{X_m}|\leq 6$, due to
 $ T_m \ncong \widetilde{\mathtt{A}}_0 $, the tree Tm has at most one claw. Moreover, in this case, Tm has no cherry and
 $ \max_{v \in \mathrm{V}_{T_m}} \deg_{T_m}(v) \leq 4 $. We thus deduce that
Tm has at most one inner vertex. This shows that
 $|{X_m}| =4$ and
 $ T_m \cong \mathrm{K}_{1,4} $.
CASE 2.2.  $ |{X_m}| \geqslant 7 $. Lines 31 to 39 of Algorithm 2 deal with this case.
We first claim that Tm has a claw. Pick  $w_1, w_2 \in \mathrm{V}_{T_m} $ such that
 $\operatorname{dist}_{T_m}(w_1,w_2)=\max\{\operatorname{dist}_{T_m}(u,v):\ u,v \in \mathrm{V}_{T_m}\setminus X_m\}$. Then, for each
 $i\in [2]$, the number of leaves of Tm contained by
 $\operatorname{N}_{T_m}(w_i)$ equals
 $\deg_{T_m}(w_i)-1$, which is at most 3. Furthermore, by Corollary 2.7 and
 $ |{\mathcal{P}^\text{cherry}_m}| \leq 1$, Tm has at most one cherry. So,
 $\operatorname{N}_{T_m}(w_1)\cap X_m$ or
 $\operatorname{N}_{T_m}(w_2)\cap X_m$ is a claw of Tm, as desired. Thanks to Lemma 4.15, the set
 $\{x,y,z\}$ defined in Line 34 is a claw of Tm. Therefore, by Lemma 3.3, Line 35 of Algorithm 2 obtains the unique phylogenetic tree Tm up to Xm-isomorphism such that
 $ \mathcal{P}_{T_m,2} = \mathcal{S}_m $.
In conclusion, Algorithm 2 outputs all phylogenetic X-trees T up to X-isomorphism such that  $ \mathcal{P}_{T,2} = \mathcal{S} $.
Proof of Theorem 1.3
(1). This is Lemma 5.1.
(2). Clearly, the score-2 split systems of two X-isomorphic phylogenetic X-trees are equal. Conversely, since one of the phylogenetic trees T and T′ is isomorphic to neither  $\mathtt{A}_0$ nor
 $ \widetilde{\mathtt{A}}_0$, by (1), the split system
 $\mathcal{P}_{T,2}=\mathcal{P}_{T',2}$ is not isomorphic to
 $\mathcal{P}_{\mathtt{A}_0,2}$. By Lemma 5.2, statement (2) now follows.
(3). Without loss of generality, assume that T′ is isomorphic to neither  $\mathtt{A}_0$ nor
 $ \widetilde{\mathtt{A}}_0$. It suffices to show that
 $\mathcal{P}_{T,2}\cong \mathcal{P}_{T',2}$ implies
 $T\cong T'$.
The condition  $\mathcal{P}_{T,2}\cong \mathcal{P}_{T',2}$ means that there exists a bijection f on X such that
 \begin{equation*}\mathcal{P}_{T',2}=\{f(A)\mid f(B):\ A\mid B\in \mathcal{P}_{T,2}\}.\end{equation*}
Let T″ be the graph with vertex set  $\tilde{f}(\mathrm{V}_T)$ and edge set
 $\{\tilde{f}(u)\tilde{f}(w):\ uw\in \mathrm{E}_T\}$, where
 \begin{equation*}\tilde{f}(v)=\begin{cases}
f(v), & \text{if } v\in X;\\
v, & \text{if } v\in \mathrm{V}_T\setminus X.
\end{cases}\end{equation*}
Clearly, T″ is a phylogenetic X-tree isomorphic to T and  $\mathcal{P}_{T^{\prime\prime},2} =\mathcal{P}_{T',2}$. Thus, by (2),
 $T'\cong_{X}T^{\prime\prime}$. Hence
 $T\cong T^{\prime\prime}\cong T'$.
6. Further research
As mentioned in the proof of Lemma 5.1,  $\mathcal{S}_{\mathtt{A}_0,2}=\mathcal{P}_{\mathtt{A}_0,2}= \mathcal{P}_{\widetilde{\mathtt{A}}_0,2}=\mathcal{S}_{\widetilde{\mathtt{A}}_0,2}$. Let
 $\{\mathtt{A}_i, \widetilde{\mathtt{A}}_i \}$,
 $i\in \{2,3,4\}$, be three additional pairs of phylogenetic trees as shown in Fig. 11. We can verify that
 $\mathcal{S}_{\mathtt{A}_i,2}= \mathcal{S}_{\widetilde{\mathtt{A}}_i,2}$ for all
 $i\in \{2,3,4\}$. In Figs. 2 and 11 we highlight some edges in green to indicate the differences between
 $\mathtt{A}_i$ and
 $\widetilde{\mathtt{A}}_i $. Similar to the pair
 $\{\mathtt{A}_{-\infty}, \widetilde{\mathtt{A}}_{-\infty} \}$ displayed in Fig. 2, these four pairs of phylogenetic trees are distinguished in Conjecture 6.1 (1), which serves as a 2-split system counterpart to Theorem 1.3 (3). Let
 $ \mathtt{B}_1, \mathtt{B}_2, \mathtt{B}_3,$ be the phylogenetic trees in Fig. 12. Conjecture 6.1 (2) is a 2-split system counterpart of Corollary 1.4.
Conjecture 6.1
Let X be a finite set, and let T and T′ be two phylogenetic X-trees.
(1) Assume that
$\{T,T'\}\notin \Bigl\{ \{\mathtt{A}_0,\widetilde {\mathtt{A}}_0\},\{\mathtt{A}_2,\widetilde {\mathtt{A}}_2\},\{\mathtt{A}_3,\widetilde {\mathtt{A}}_3\}, \{\mathtt{A}_4,\widetilde {\mathtt{A}}_4\} \Bigr\}$. Then,
$\mathcal{S}_{T,2} \cong \mathcal{S}_{T',2}$ if and only if
$ T \cong T' $.(2) Assume that
$\mathcal{S}_{T,2}=\mathcal{S}_{T',2}$ and
$T\ncong_X T'$. Then, T and T′ are isomorphic if and only if they are both isomorphic to a common member of
$ \widetilde{\mathtt{A}}_0, \widetilde{\mathtt{A}}_3, \widetilde{\mathtt{A}}_4, \mathtt{B}_1, \mathtt{B}_2, \mathtt{B}_3$.


Three pairs of trees with isomorphic 2-split systems. (A)  $\mathtt{A}_2$, (B)
 $\mathtt{A}_3$, (C)
 $\mathtt{A}_4$, (D)
 $\widetilde{\mathtt{A}}_2$, (E)
 $\widetilde{\mathtt{A}}_3$, (F)
 $\widetilde{\mathtt{A}}_4$

Three binary trees. (A)  $\mathtt{B}_1$, (B)
 $\mathtt{B}_2$, (C)
 $\mathtt{B}_3$

We will prove Conjecture 6.1 in [Reference Qian, Wu and Xie62]. This paper is concerned with score-2 split systems while [Reference Qian, Wu and Xie62] is devoted to 2-split systems. It is thus not surprising that in [Reference Qian, Wu and Xie62] we also need Algorithm 1 and we have a counterpart of Lemma 4.4 as a basic lemma there.
Let  $ \ell\geqslant 2 $ be an integer. Wilde and Fischer [Reference Wilde and Fischer69, Corollary 3] presented two phylogenetic
 $[2\ell +2]$-trees T 1 and
 $ T_1' $ satisfying
 $ \mathcal{P}_{T_1,\ell}=\mathcal{P}_{T_1',\ell} $ which are isomorphic but not
 $[2\ell +2]$-isomorphic. In Conjecture 6.2 (5), we further claim that there exist non-isomorphic phylogenetic
 $[2\ell +2]$-trees T 1 and
 $ T_1' $ such that
 $ \mathcal{P}_{T_1,\ell}=\mathcal{P}_{T_1',\ell} $. Wilde and Fischer [Reference Wilde and Fischer70, Theorem 5] proved that, for every
 $ |X| \geqslant 2 \ell + 3 $ and every two binary phylogenetic X-trees T 1 and
 $ T_1' $,
 $ \mathcal{P}_{T_1,\ell}=\mathcal{P}_{T_1',\ell} $ implies that T 1 and
 $ T_1' $ are X-isomorphic. Conjecture 6.2 (4) is a generalization of this result to non-binary case. We report analogous results in Conjecture 6.2 (1), (2) and (3).
Conjecture 6.2
Let  $\ell$ be a positive integer, and let X be a finite set. When
 $ \ell \geqslant 2 $, let
 $ X_\ell \doteq \{x_1,\dots,x_{\ell+2}, y_1,\dots,y_{\ell+2}\} $ be a set of size
 $2\ell+4$, and, for every
 $ j \in [\ell] $, let
 $ T_{\ell,j} $ be the
 $X_\ell$-tree shown in Fig. 13. Note that
 $ T_{\ell,j} $ and
 $ T_{\ell,j'} $ are non-isomorphic for all
 $ \{j,j'\} \in \binom{X_\ell}{2} $.
 $\ell$ trees T sharing the same
 $ \mathcal{P}_{T,\leq \ell} $ and the same
 $ \mathcal{P}_{T,\ell + 1} $, where
 $ \ell \geqslant 2 $. (A) Trees
 $ T_{\ell,m} $, where
 $ m-1 \in [\ell -1 ] $. (B) The tree
 $ T_{\ell,1} $.

(1) If
$|X|\geqslant 2\ell+5$, then two phylogenetic X-trees T and T′ are X-isomorphic if and only if
$\mathcal{S}_{T,\ell}=\mathcal{S}_{T',\ell}$.(2) If
$|X|\geqslant 2\ell+5$, then two phylogenetic X-trees T and T′ are X-isomorphic if and only if
$\bigcup_{0\leq i\leq \ell}\mathcal{P}_{T,i}=\bigcup_{0\leq i\leq \ell}\mathcal{P}_{T',i}$.(3) If
$ \ell \geqslant 2 $, then
$ |{X_\ell}| = 2\ell+4 $, the phylogenetic
$X_{\ell}$-trees
$T_{\ell,j}$,
$ j \in [\ell ] $, are pairwise non-isomorphic, but
$ \bigcup_{0\leq i\leq \ell}\mathcal{P}_{T_{\ell,j},i} $ is a split system independent of
$ j \in [\ell ] $.(4) If
$|X|\geqslant 2\ell+3$, then two phylogenetic X-trees T and T′ are X-isomorphic if and only if
$\mathcal{P}_{T,\ell}=\mathcal{P}_{T',\ell}$.(5) If
$\ell\geqslant 3$, then
$ |{X_{\ell-1}}| = 2\ell+2 $ and the phylogenetic
$X_{\ell-1}$-trees
$T_{\ell-1,j}$,
$ j \in [\ell-1] $, are pairwise non-isomorphic but share a common score-
$\ell$ split system.


We have verified Conjecture 6.2 (1) and we plan to further study if the bound of  $|X|\geqslant 2\ell+5$ there is sharp before completing the corresponding paper. We will prove Conjecture 6.2 (2) and (3) in [Reference Qian, Wu and Xie63], and Conjecture 6.2 (4) and (5) in [Reference Qian, Wu and Xie64].
In order to tell a tree from its score-2 split system, one important step in our work is to tell a vertex of large degree; see Case 1 of the proof of Lemma 5.2 (2). To extend this step for the recognition of large degree vertex from general score- $\ell$ split systems, we propose Conjectures 6.3 and 6.4. Note that both conjectures hold true when
 $\ell=2$, as guaranteed by Corollary 4.8, Corollary 4.10 (2) and Lemma 4.13.
Conjecture 6.3
Let k and  $ \ell $ be two integers such that
 $ k \geqslant \ell+3 \geqslant 5 $. Let T be a phylogenetic tree, and take
 $ Y\mid (\mathrm{L}_T\setminus Y) \in \mathcal{P}_{T,\ell} $. Assume that
 $\pi= Y_1 \mid \dots \mid Y_k $ is a k-partition of Y such that
 $ \Gamma_{\mathcal{P}_{T,\ell}}(Y) = \operatorname{\mathcal{H}}_{\pi, \ell }$, namely, Y is a
 $(k,\ell)$-set with respect to
 $ \mathcal{P}_{T,\ell}$. Then, there exists a unique
 $ v \in \mathrm{V}_T $ such that the connected components of T − v can be enumerated as
 $ V_1, \ldots, V_{k+\ell} $ with
 $ V_i \cap \mathrm{L}_T = Y_i $ for all
 $ i \in [k] $.
Conjecture 6.4
Let k and  $ \ell $ be two integers such that
 $ k \geqslant \ell+1 \geqslant 3 $, and let T be a phylogenetic tree. Assume that
 $T\ncong \widetilde{\mathtt{A}}_0$. Let
 $\pi= Y_1 \mid \dots \mid Y_{k+\ell} $ be a
 $(k+\ell)$-partition of
 $ \mathrm{L}_T $ such that
 $ (\bigcup_{i \in I} Y_i) \mid (\bigcup_{i \in [k+\ell] \setminus I} Y_i) \in \mathcal{P}_{T,\ell} $ and
 $ \Gamma_{\mathcal{P}_{T,\ell}}(\bigcup_{i \in [k+\ell] \setminus I} Y_i) = \{\bigcup_{i \in I'} Y_i : I' \in \binom{[k+\ell]\setminus I}{\ell}\} $ for every
 $ I \in \binom{[k+\ell]}{\ell} $. Then, there exists a unique
 $ v \in \mathrm{V}_T $ that allows us to enumerate the connected components of T − v as
 $ V_1, \ldots, V_{k+\ell} $ such that
 $V_i \cap \mathrm{L}_T = Y_i $ for all
 $ i \in [k+\ell] $.
Buneman graphs and Buneman complexes have been useful tools for visualizing split systems [Reference Besenbacher, Mailund, Westh-Nielsen and Pedersen8, Reference Buneman, Hodson, Kendall and Tautu12, Reference Choe, Huber, Koolen, Kwon and Moulton18, Reference Dress, K. T., Huber and Moulton25, Reference Dress, Huber, Koolen, Moulton and Spillner27–Reference Dress, Huber and Moulton29, Reference Misra, Blelloch, Ravi and Schwartz57]. The Buneman Theorem concerning 1-split systems, namely Theorem 1.1, can be proved using the Buneman graph. It is reasonable to expect that a similar approach could be applied to directly reconstruct a tree from a suitable k-split system or score-k split system. Below, we outline one such possible procedure. Let X be a finite set, let  $ \mathcal{S} $ be a split system over X, and let
 $\ell$ be a positive integer. Let
 $\mathrm{V}_\ell (\mathcal{S})$ be the set of all functions
 $ f: \ \mathcal{S} \to 2^X $ satisfying the following two conditions:
(1) The condition
$f(\mathbf{S})\in \mathbf{S}$ holds for all
$\mathbf{S} \in \mathcal{S}$.(2) The intersection
$ \bigcap_{\mathbf{S}\in \mathcal{S}'} f(\mathbf{S}) \neq \emptyset $ holds for every
$\mathcal{S}' \in \binom{\mathcal{S}}{\ell} $.


We define the  $\ell$th generalized Buneman graph, denoted by
 $ \operatorname{B}_{\ell}(\mathcal{S}) $, as the graph with vertex set
 $\mathrm{V}_\ell (\mathcal{S})$ and with
 $uv\in \binom{\mathrm{V}_\ell (\mathcal{S})}{2}$ being an edge of
 $ \operatorname{B}_{\ell}(\mathcal{S}) $ exactly when the Hamming distance between u and v is the smallest among all pairs of distinct elements from
 $\mathrm{V}_\ell (\mathcal{S})$. Note that what is known as the Buneman graph [Reference Buneman, Hodson, Kendall and Tautu12, p. 388] [Reference Dress, Huber and Moulton28, § 4.1] in the literature corresponds to our
 $ \operatorname{B}_{2}(\mathcal{S}) $. For every positive integer
 $\ell$, let
 $\delta_\ell$ denote the smallest positive integer d such that
 $ \operatorname{B}_{\ell+1}(\mathcal{S}_{T,\ell})\cong T $ for every tree T with at least three vertices whose inner vertices have degrees no smaller than d; let
 $\delta'_\ell$ denote the smallest positive integer d such that
 $ \operatorname{B}_{\ell+1}(\mathcal{P}_{T,\ell})\cong T $ for every tree T with at least three vertices whose inner vertices have degrees no smaller than d. When Buneman [Reference Buneman, Hodson, Kendall and Tautu12, p. 389] used the Buneman graph to establish Theorem 1.1, what he actually proved is just
 $\delta_1= \delta'_1=3$.
Conjecture 6.5
(1) For every positive integer  $\ell$, we have
 $\infty \gt \delta_\ell=\delta'_\ell \gt 2\ell$. (2)
 $\delta_2= \delta'_2 =7$.
Question 6.6. Let T be a phylogenetic tree, let  $\ell$ be a positive integer, let
 $\mathbf{S} \in \mathcal{S}_{T,\ell}$ and let
 $\mathcal{S}$ be the full
 $\ell$-split system of T induced by S. When is
 $\mathcal{S}$ compatible? When
 $\ell=1$,
 $\mathcal{S}$ is a singleton set and hence compatible. When
 $\ell =2$, the compatibility of
 $\mathcal{S}$ is ensured by Lemma 2.10. Note that compatible split systems arise in Buneman theorem (Theorem 1.1 (1)) and Apresjan’s Lemma [Reference Dress, Huber and Moulton28, Lemma 7.5].
Though a split can be considered an unoriented/affine object, it has a close relationship with its oriented/projective counterparts [Reference Dasarathy, Mossel, Nowak and Roch20, Reference Dress, Klucznik, Koolen and Moulton30, Reference Koloschin, Krill and Pitz51]. Split systems, as well as the similar concept of separation systems – particularly those with tree-like behaviours – have been an important research subject in geometric group theory [Reference Adam-Day1, Reference Elbracht, Kneip and Teegen33, Reference Tserunyan68], cluster algebra [Reference Danilov, Karzanov and Koshevoy19, Reference Gambette, Huber and Scholz41], electrical networks [Reference Francis, Huber, Moulton and Wu39], random processes [Reference Fischer35, Reference Steel67], structural graph theory and matroid theory [Reference Bowler and Kneip11, Reference Diestel, Hundertmark and Lemanczyk22, Reference Evans34, Reference Gioan and Paul42, Reference Goloboff and Wilkinson43, Reference Kupavskii, Pach and Tomon52, Reference Oum59, Reference Schröter65], extremal set theory [Reference Dunwoody and Krön32, Reference Li, Fan, Ito, Karimi and Xu53], and cluster analysis and phylogenetic combinatorics [Reference Buneman, Hodson, Kendall and Tautu12, Reference Dress, Hendy, Huber and Moulton26, Reference Dress, Huber and Moulton28, Reference Hellmuth, Schaller and Stadler45–Reference Helminck47, Reference Huber, Moulton, Semple and Wu49]. It seems promising to further expand our current work to the setting of other mathematical contexts, such as any of the above-mentioned ones.
Splits are very special partitions. What are the partition counterparts for Theorem 1.3, conjectures 6.1 and 6.2? Note that, in biology, a character is a partition of a subset of species. We refer to [Reference Aliste-Prieto, Martin, Wagner and Zamora3, Reference Bordewich, Deutschmann, Fischer, Kasbohm, Semple and Steel9, Reference Bordewich, Semple and Steel10, Reference Kleinman, Harel and Pachter50, Reference Orellana and Scott58, Reference Steel67] for some interesting study of partitions from tree structures. For a tree T, the splits of  $\mathrm{L}_T$ discussed in this paper are related to unions of one or two convex sets in T. It would be intriguing to explore how to advance this research in an extended study of abstract convexity [Reference Bordewich, Deutschmann, Fischer, Kasbohm, Semple and Steel9, Reference Bertrand and Diatta7, Reference Cantone, Doignon, Giarlotta and Watson14, Reference Chalopin, Chepoi and Giocanti16, Reference Develin and Sturmfels21, Reference Petrov60].
Acknowledgements
The thorough review from our referees had a profound impact on improving the quality of the presentation of this paper. This work was supported by the Fundamental Research Funds for the Central Universities. We dedicate this paper to the memory of Andreas Dress (26 August, 1938–23 February, 2024), who worked from 2005 to 2010 in the Life Science Building at Yueyang Road 320, Shanghai. From 1946 to 1948, Shiing-Shen Chern (26 October, 1911–3 December, 2004) also worked in the same building. Wenjun Wu, a distinguished alumnus of Jiao Tong University, followed Chern to study algebraic topology at Yueyang Road 320 during that time; according to his recollections, Chern’s office was located on the second floor. We have vivid memories of the third floor, particularly room 305 (Dress’s office), the seminar room, and the common room. It was through interactions with individuals who frequented the third floor, including Dress and his colleagues, that we gained a foundational understanding of the intrinsic beauty of trees.



