In dairy cows only about 20% of the milk is stored in the cisternal cavity and is directly available before milk ejection (Bruckmaier et al. Reference Bruckmaier, Rothenanger and Blum1994b; Pfeilsticker et al. Reference Pfeilsticker, Bruckmaier and Blum1996; Ayadi et al. Reference Ayadi, Caja, Such and Knight2003, Reference Ayadi, Caja, Such, Rovai and Albanell2004). The main portion of the milk is located in the alveoli and small milk ducts and can be extracted only after milk ejection has shifted it into the cistern. The induction of milk ejection requires tactile stimulation of the teats and/or the udder which causes the release of oxytocin and hence myoepithelial contraction and alveolar milk ejection (Bruckmaier & Blum, Reference Bruckmaier and Blum1996; Bruckmaier, Reference Bruckmaier2005). Pre-stimulation induces the milk ejection already before the start of milking, whereas milking without pre-stimulation leads to a transient reduction (bimodality) of milk flow after removal of the cisternal milk and before the availability of alveolar milk which is ejected in response to the stimulation by the teat cup liner during the normal milking procedure (Schams et al. Reference Schams, Mayer, Prokopp and Worstorff1984; Bruckmaier & Blum, Reference Bruckmaier and Blum1996; Weiss et al. Reference Weiss, Dzidic and Bruckmaier2003; Sandrucci et al. Reference Sandrucci, Tamburini, Bava and Zucali2007). Milk ejection continues throughout the whole milking (Bruckmaier et al. Reference Bruckmaier, Schams and Blum1994a; Weiss et al. Reference Weiss, Dzidic and Bruckmaier2003) and, towards the end of milking, the transfer of milk into the cistern can be a limiting factor for the milk flow rate (Pfeilsticker et al. Reference Pfeilsticker, Bruckmaier and Blum1995).
Peak milk flow rate (PFR) can be modified by changes of the pulsation ratio (Pfeilsticker et al. Reference Pfeilsticker, Bruckmaier and Blum1995; Hamann & Mein, Reference Hamann and Mein1996). The same is true to a limited extent for the average milk flow (AMF) and consequently for the total milking time. While a higher PFR does not necessarily mean a faster udder emptying throughout the milking process, a higher AMF leads to a shorter total milking time at a given amount of milk stored in the udder (Smith & Petersen, Reference Smith and Petersen1946; Thomas et al. Reference Thomas, Force, Bremel and Strasser1991; Pfeilsticker et al. Reference Pfeilsticker, Bruckmaier and Blum1995; Gleeson et al. Reference Gleeson, O'Callaghan and Rath2004).
The objective of this present study was to test the hypothesis that milking with milk flow-controlled changes of the b-phase of the pulsation lead to a faster milk removal than standard pulsation which remains unchanged throughout milking.
Materials and Methods
Animals and housing
Twenty-nine Holstein cows in early (7), mid (14) and late (8) lactation from a private farm in Switzerland were used (early: 1–100 d post partum (p.p.), mid: 101–200 d p.p., late lactation: 200–370 d p.p.). During the experiment the cows were in their first (9), second (2), third (9), fourth (7), sixth (1) and seventh (1) lactations.
Mean 305-d milk-production was 8945 kg and ranged from 5095 kg to 10 968 kg in the preceding lactation of the 20 multiparous cows. The animals were kept in a loose housing stall on cleft floor and fed with 40% maize silage, 10% sugar beet silage, 35% green silage, 8% hay and concentrate (approximately 7% soy pellets and a cereal mix), according to their individual production levels.
Milking and milk-flow recording
Cows were milked in a low-level 1×6 side-by-side-milking parlour with a Lemmer-Fullwood SBS Arizona Group MM95 CE (6344 Meierskappel, Switzerland) at a vacuum level of 40·5 kPa and with a 4×1 pulsation. Times of milking were in the morning from 5·45 (i.e. 13 h after previous milking) and in the evening from 16·45 (i.e. 11 h after previous milking). All milkings were performed by the same person. The liner used was a Lemmer-Fullwood CTF 720138 (6344 Meierskappel, Switzerland).
The experiment included 18 milkings (9 d) and milk flow curves of all milkings were recorded with mobile milk-flow recording units (LactoCorder®, WMB AG, 9436 Balgach, Switzerland).
Udder preparation, pre-stimulation and milking routine (PS+):
The milker wore Nitril gloves during milking. After entering the parlour teats of all cows were foamed with Dermaline (5–20% anionic surfactant, 1–5% glycerol, 1–5% anionic tenside, perfume and triclosan; CID LINES NV/SA, 8900 Ieper, Belgium) and thereafter dried with a single-use paper. Subsequently the clusters were attached without pre-stripping. The process of this routine was always similar and lasted 50–70 s from the first touch of the udder until cluster attachment. After cluster attachment a 35-s high-frequency pre-stimulation was applied (pulsation rate: 250 cycles/min; pulsation ratio: 25:75). As soon as the metering box was not completely filled within 35 s (i.e. <200 g milk within 35 s) the clusters were removed automatically with a delay of about 1 s.
Milk flow controlled b-phase (MB+):
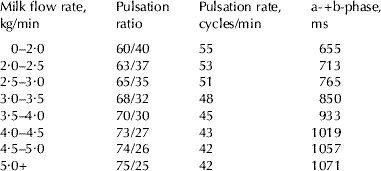
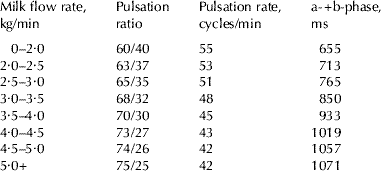
The milking machine used was equipped with a special option to adjust the b-phase of the pulsation on the basis of the current milk flow rate as shown in Table 1. This adjustment caused changes of pulsation ratio and pulsation rate. Overall the adjustments cause longer liner-open periods during phases with high milk flow. A-, c- and d-phases of the pulsation curve remained unchanged.
The milking machine settings and their changes when milked with milk flow-controlled b-phase
Treatments
PS+/MB−:
In this treatment the pulsation ratio was 60:40 and the pulsation rate was 55 cycles/min which remained unchanged throughout the entire milking. Cows were milked with the usual milking routine and without milk flow-controlled b-phase on days 2, 6 and 9 of the study.
PS+/MB+:
The routine udder preparation was performed and the cows were milked with milk flow-controlled b-phase on days 3, 5 and 8.
PS−/MB−:
This treatment included a minimum of teat cleaning. First the teats of all 6 cows in the parlour were foamed, then one cow after the other was cleaned within some seconds with a single-use paper and the cluster was attached immediately. Milking was performed without milk flow-controlled b-phase. The clusters were removed automatically. This treatment was used on days 1, 4 and 7 of the study.
Milking characteristics
During all experimental milkings the milking characteristics as calculated by the LactoPro Software (Version 5.2.0 Beta 49 software; WMB AG, 9436 Balgach, Switzerland, 2007) were used for evaluation of milk flow curves. The parameters used were total milk yield (TMY), main milking time 1 (MMT1, time from milk flow >0·5 kg/min at the start of milking until <0·2 kg/min at the end of milking), peak flow rate (PFR, highest milk flow, which is maintained for at least 22 s), time until peak flow rate (tPFR), average milk flow during MMT1 (AMF), duration of incline (dI, duration from a milk flow of 0·5 kg/min at the start of milking until milk flow reached a plateau, i.e. the slope of the increasing milk flow reached a threshold of <0·8 kg/min2), duration of plateau (dP, after incline until milk flow dropped to a slope of >0·8 kg/min2) and duration of decline (dD, after plateau until 0·2 kg/min) and the occurrence of bimodal milk flow (BIMO, milk flow >0·5 kg/min, a decline of >0·2 kg/min and an increase of >0·5 kg/min within 38 s after the decline).
An additional parameter not included in the LactoPro software was introduced. Main milking time 2 (MMT2, time recorded from >0·5 kg/min until <0·5 kg/min) was used to detect a potential treatment effect on milking time if the cluster would be removed at a higher milk flow level. MMT2 was calculated manually from the milk flow curves.
Mathematical and statistical evaluations
The herd was subdivided into three groups based on the individual peak flow rate in the treatment PS+/MB−. In group 1 the PFR was <3·2 kg/min, in group 2 between 3·2 and 4·5 kg/min, and in group 3 >4·5 kg/min.
All data are presented as means and sem for the herd, for each group separately and for the different treatments. For the statistical evaluation a Mixed Procedure of SAS (Release 8.02) was used. The model contained the treatment, time of milking, stage of lactation, animal group and the individual cow as the repeated subject. None of the interactions included in the model (treatment×animal group, treatment×milking time and treatment×stage of lactation) were significant. They were therefore excluded from the model. Differences of least squares means were localized by t test and considered significant if P<0·05. Treatment differences with respect to the frequency of occurrence of bimodalities were tested for significance (P<0·05) by using a Multtest Procedure of SAS.
Results
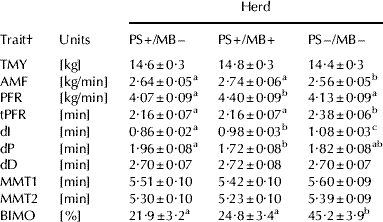
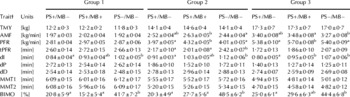
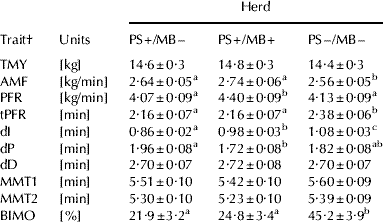
TMY did not differ significantly between treatments (Tables 2, 3). In group 1 TMY was lower than in group 2 and than in group 3, and the value in early lactation was higher than mid and late lactation, and mid was higher than late lactation (P<0·05). At morning milking TMY was significantly higher than at evening milking at a herd level and in all groups. In group 1 TMY was significantly lower in early and late compared with mid lactation. In group 2 TMY was higher in early than in mid and late lactation (P<0·05). If all experimental animals were considered, AMF was significantly lower in PS−/MB− than in PS+/MB− and PS+/MB+. PS+/MB+ had the highest values. In group 1 AMF was significantly lower than in groups 2 and 3, in group 2 AMF was lower than in group 3. At a herd level, AMF was higher in early lactation than in mid and late lactation, and in mid lactation AMF was higher than in late lactation (P<0·05). Within groups 2 and 3 AMF was higher (P<0·05) in PS+/MB+ than in PS−/MB−. In group 1 no significant difference could be observed. Although differences were often non-significant, highest values of AMF were observed in all animal groups (groups 1, 2, 3 and the herd) in treatment PS+/MB+, followed by PS+/MB− and PS−/MB− (Tables 2, 3). AMF was significantly lower in early and late compared with mid lactation in group 1 (P<0·05). In group 2 AMF was lower in early than in mid and late lactation, and in group 3 AMF was highest for early compared with mid and finally late lactation (P<0·05). At morning milking AMF was significantly higher at a herd level and in all groups.
Milk flow traits of different treatments in the herd
abc Values in the same row without common superscript are significantly different (P<0·05)
† See text for definitions of abbreviations
Milk flow traits of different treatments in different groups

ab Values in the same group without common superscript are significantly different (P<0·05)
† See text for definitions of abbreviations
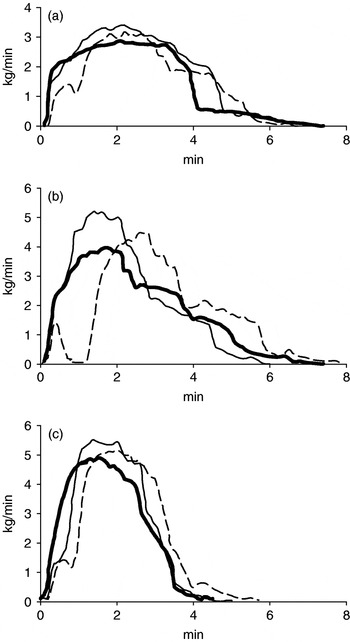
PFR was significantly higher (Fig. 1) in treatment PS+/MB+ than in the other treatments in groups 2 and 3. PFR in treatments PS+/MB− and PS−/MB− did not differ significantly. Only in group 1, the cows with the lowest PFR (<3·2 kg/min), PFR did not significantly differ between any treatments (Tables 2, 3). PFR was lower in group 1 than in group 2 and group 3, respectively. PFR was higher at morning than at evening milkings and higher in early and mid compared with late lactation (P<0·05). In group 2 PFR was significantly lower in early than in mid and late lactation and PFR was significantly higher in early compared with mid and compared with late lactation.
Milk flow curves of a cow of group 1=PFR<3·2 kg/min (a), of group 2=PFR 3·2–4·5 kg/min (b) and of group 3=PFR>4·5 kg/min (c) with the different treatments (PS+/MB−:  ; PS+/MB+: —; PS−/MB−: – –). PS: pre-stimulation; MB: milk flow-controlled b-phase.

tPFR was significantly longer in group 2 in PS−/MB− compared with the other treatments (Table 3). tPFR was longer in group 1 compared with groups 2 and 3 and in group 2 compared with group 3 (P<0·05). tPFR was higher in early and mid lactation than in late lactation (P<0·05). tPFR was significantly shorter in early than in mid and late lactation in group 1. In group 3 tPFR was significantly higher in early and mid lactation compared with late lactation.
Duration of incline over the whole herd was significantly different between all treatments. dI was longer in group 2 compared with groups 1 and 3 and it was shorter during evening than morning milkings (P<0·05). A significant difference was seen in groups 1 and 2 between PS−/MB− and PS+/MB− and in group 3 in PS+/MB− compared with PS−/MB− and PS+/MB+. In all groups and consequently over the whole herd, dI was shortest in PS+/MB−, followed by PS+/MB+ and PS−/MB− (Tables 2, 3). In group 1 dI was longer for early and late lactation compared with mid lactation, whereas in group 2 dI was higher at evening than morning milkings (P<0·05). dI was shorter in early and mid lactation than in late lactation in group 2 and in group 3 it was longer for early and mid compared with late lactation (P<0·05).
Both duration of plateau (dP) and duration of decline (dD) did not significantly differ among the treatments. Except for the herd, dP was significantly longer for PS+/MB+ than PS+/MB−. dP was longer in group 1 than in group 2 and than in group 3 (P<0·05). dD was shorter in group 1 than in group 2 and for early lactation dP was higher than mid and late lactation, and mid was higher than late lactation (P<0·05). At evening milkings dP was always significantly shorter for all animals and for all groups. In group 1 dP was significantly longer in early than late lactation, in group 2 it was significantly shorter in early than in mid and late lactation, and in group 3 it was significantly longer in early compared with mid and at the end late lactation. dD was shorter in early and mid lactation compared with late lactation for group 1, while in group 2 dD was higher in early compared with mid and late lactation and in group 3 it was shorter for early and late lactation as compared with mid lactation (P<0·05).
MMT1 and MMT2 were not significantly different between the different treatments (Fig. 1). In all groups (except for MMT2 in group 2) and over the whole herd both parameters were numerically shortest in PS+/MB+, followed by PS+/MB− and then PS−/MB− (Tables 2, 3). MMT1 and MMT2 were longer in group 1 compared with group 2 and at the end group 3, and in early lactation they were longer than in mid and late lactation and mid were longer than late lactation (P<0·05). MMT1 and MMT2 were significantly shorter during evening than during morning milkings at a herd level and all groups except for MMT1 in group 2. In group 2 MMT1 and MMT2 were longer for early compared with mid and late lactation and in group 3 they were longer for early and mid compared with late lactation (P<0·05).
Bimodality was most frequent in PS−/MB− followed by PS+/MB+ (except group 1) and PS+/MB− (Fig. 1). In group 1 the frequency of bimodality was significantly higher in PS−/MB− than in PS+/MB− and PS+/MB+. In group 2 and over the whole herd it was higher in PS−/MB− than in PS+/MB+ and PS+/MB− (P<0·05). In group 3 it was significantly more frequent in PS−/MB− than in PS+/MB−.
Discussion
TMY did not change throughout the experiment. This indicates complete emptying of the mammary gland in every treatment and for every group.
AMF did not differ between treatments in all groups (except in group 2 between PS+/MB+ and PS−/MB−). Thus, even if there was a higher PFR in all observed groups and all over the groups (herd) AMF and TMY remained unchanged. This is in contrast to the report by Spencer et al. (Reference Spencer, Shin, Rogers and Cooper2007), where AMF augmented with elevating ratio. Obviously, the milk ejection rate, i.e. the rate of milk transferred from the alveolar tissue into the cisternal cavities, is a limiting factor for the milk flow rate (Pfeilsticker et al. Reference Pfeilsticker, Bruckmaier and Blum1995). At the start of milking the cistern is well filled with milk and the milk ejection rate is high owing to well-filled alveoli. Therefore, the milk flow rate during this period is mainly determined by the teat anatomy and specifications of liner, pulsation, and vacuum (Thomas et al. Reference Thomas, Force, Bremel and Strasser1991; Pfeilsticker et al. Reference Pfeilsticker, Bruckmaier and Blum1995; Hamann & Mein, Reference Hamann and Mein1996; Weiss et al. Reference Weiss, Weinfurtner and Bruckmaier2004; Spencer et al. Reference Spencer, Shin, Rogers and Cooper2007). In contrast, towards the end of milking, the delivery of milk from the secretory tissue in the cistern is slowing down owing to the gradual emptying of the alveoli, i.e. the milk ejection rate is decreasing. This process cannot be influenced by adjustments of the milking machine and the milk ejection rate can be a major limiting factor for the milk flow towards the end of milking, and a flat decline of milk flow in each quarter probably represents the decline of milk ejection (Pfeilsticker et al. Reference Pfeilsticker, Bruckmaier and Blum1995). In PS+/MB+ peak flow rates were higher than in PS−/MB− or in PS+/MB−. If milking was performed with milk flow-controlled b-phase (PS+/MB+) the pulsation ratio increased and the pulsation rate declined, causing an overall elongated liner-open time if ample milk was present in the cisternal cavities. As long as this situation was maintained, the milk flow rate could be increased in response to a longer liner-open phase. Potentially it is possible that the increase in milk flow could prevent the liner from closing and could cause oedema. But high milk flow lasts only about 2–3 min and then the machine is already changing the pulsation ratio and rate, and therefore there would be minimal oedema. Milking with milk flow-controlled b-phase is even more gentle on the teat because of the changing pulsation ratio and rate. Owing to the increase of the pulsation ratio, PFR soars as long as a buffer of milk is available in the cistern (Pfeilsticker et al. Reference Pfeilsticker, Bruckmaier and Blum1995; Hamann & Mein, Reference Hamann and Mein1996; Spencer et al. Reference Spencer, Shin, Rogers and Cooper2007). tPFR occurred later (except for group 2) and dI was longer than can be explained by a higher level of PFR which needed to be reached stepwise in the treatment with gradually elongated b-phase. Because TMY and AMF did not change a lot between the different treatments, MMT1 remained unchanged (MMT1 lasted until 0·2 kg/min). If the milk ejection rate becomes limiting for milk flow towards the end of milking, it seems possible that the final period of milking at very low milk flow rates <0·5 kg/min has a great effect on the remaining milking time. Therefore a difference between treatments seemed possible if the clusters would be removed already at 0·5 kg/min (MMT2). However, also at this higher level of potential cluster removal no treatment differences were observed. Bimodality of milk flow was most frequent in PS−/MB−. This is allegedly due to a delayed occurrence of milk ejection while the cisternal milk is close to being completely removed. As repeatedly shown (Mayer et al. Reference Mayer, Schams, Worstorff and Prokopp1984; Bruckmaier & Blum, Reference Bruckmaier and Blum1996; Weiss et al. Reference Weiss, Dzidic and Bruckmaier2003) a not-fully pre-stimulated cow shows a transient reduction of milk flow (bimodality), after the cisternal part is milked out and before the milk ejection occurs.
Effects on PFR and dI were more distinct in the two groups with higher PFR (groups 2 and 3) than in the group with the lowest PFR (group 1).
In conclusion, adaptation of the b-phase on the milk flow (PS+/MB+) causes an increased milk flow rate most pronounced in animals that already show high milk flow rate under standard conditions. This effect is, however, only present as long as milk is available in the cisternal cavities. In particular, towards the end of milking the rate of milk ejection can become a limiting factor for milk flow. During this period, an adaptation of the b-phase on the milk flow (PS+/MB+) has no effect. Therefore, the performed adaptations (PS+/MB+) have mainly an effect on PFR and not on AMF and total milking time.
Bimodality was most frequently seen in milking with a minimum of teat cleaning and without milk flow controlled b-phase (PS−/MB−).