Implications
In pig litters of normal size (10 to 15 pigs), large differences in average litter weight are generally observed. The question arises whether offspring born from normal litter size but classified as having lower than average litter birth weight suffered an intrauterine insult. The observed greater number of stillborns and higher pre-weaning mortality is indicative of impaired prenatal development of these littermates. Despite post-weaning catch-up growth found in offspring born from low birth weight litters, increasing average litter weight should be targeted to enhance sow reproduction performance and offspring viability.
Introduction
In the last 10 years, sow prolificacy markedly increased in many pig breeds as, for instance, the Swiss Large White populations (Suisag, 2012). With a litter size ranging from 5 to 20 piglets born, a distinct linear decrease in average litter birth weight and a concomitant increase in the proportion of low birth weight pigs can be observed (Foxcroft et al., Reference Foxcroft, Bee, Dixon, Hahn, Harding, Patterson, Putman, Sarmento, Smit, Tse and Town2007; Fix et al., Reference Fix, Cassady, Holl, Herring, Culbertson and See2010). Although average litter birth weight is still moderately inverse to litter size when only litters with 10 to 15 newborns are included in the analysis (Foxcroft et al., Reference Foxcroft, Bee, Dixon, Hahn, Harding, Patterson, Putman, Sarmento, Smit, Tse and Town2007), the between-litter variance in average litter birth weight can still reach a maximum of 1 kg. These observations led to the assumption that different patterns of prenatal losses in gestating sows may cause differences in average litter birth weight. On the basis of the compelling evidence delivered by van der Waaij et al. (Reference van der Waaij, Hazeleger, Soede, Laurenssen and Kemp2010), greater mortality rates between implantation on day 13 and up to day 40 of pregnancy had detrimental effects on placenta weight, thus impairing development of the fetuses.
Impaired placental efficiency is predicted to result in prenatal programming effects not only of individual pigs but, to some extent, of all offspring in the litter (Wu et al., Reference Wu, Bazer, Wallace and Spencer2006; Foxcroft et al., Reference Foxcroft, Bee, Dixon, Hahn, Harding, Patterson, Putman, Sarmento, Smit, Tse and Town2007). Because the early stages of gestation mark the onset of myogenesis (Zhao et al., Reference Zhao, Mo, Li, Gong, Xiao, Zhang, Qin, Niu, Guo, Liu, Cong, He, Wang, Li and Chen2011), it is reasonable to assume that differences in placental efficiency caused by different prenatal survival patterns will affect myogenesis and ultimately postnatal growth efficiency (Dwyer et al., Reference Dwyer, Fletcher and Stickland1993).
On the basis of these assumptions, the aim of the study was to compare litter characteristics, as well as postnatal growth performance, carcass characteristics and meat quality traits of offspring originating from litters with 10 to 15 pigs born with either high- or low-average litter birth weight. Of special interest was the question of how the assumed different pattern of prenatal losses could affect postnatal development of the progeny. Therefore, pigs of both genders that (1) either fell within the mid-birth weight range of their respective litters in the two average birth weight groups or (2) had a similar birth weight but originated from different average litter birth weight groups were investigated.
Material and methods
Animals and treatments
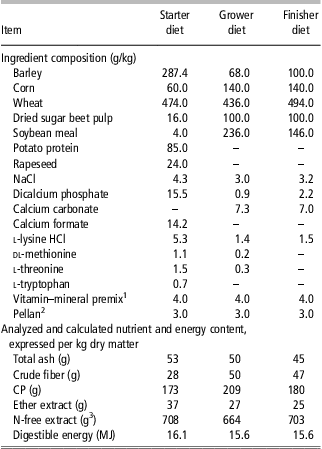
All procedures involving animals were approved by the Swiss Cantonal Committee for Animal Care and Use. From the herd of the Agroscope Liebefeld Posieux research station, a total of 16 multiparous Swiss Large White sows (parity 2 to 6) were selected. Two criteria were considered for sow selection: (1) the number of piglets born per litter had to be in the range of 10 to 15 piglets and (2) the average litter birth weight had to be either >1.7 kg (H) or<1.3 kg (L). Allocation to these two treatment groups was performed on the day of farrowing considering the number of total piglets born and the average litter birth weights. Sows were artificially inseminated three times on 2 consecutive days with unfrozen semen from 10 Swiss Large White boars (Suisag, Sempach, Switzerland). During the gestation and lactation periods, all sows were fed standard diets formulated according to Swiss nutrient recommendations for pigs (Agroscope Liebefeld Posieux Research station (ALP), 2012). Within 12 h after birth, the number of piglets born alive, the number of stillborn and their individual BW were determined. As requested by the Swiss animal welfare law, male pigs were castrated only after isoflurane anesthesia induction within 4 days after birth. All piglets of the H- and L-sows stayed with the dam until weaning at day 27 (±1.2 days), and no cross-fostering was permitted. Suckling piglets had access to creep feed from day 10 until the end of lactation. At weaning, where available, two castrates and two female pigs were chosen from each litter for assessing growth performance during the starter and grower–finisher periods and carcass characteristics and meat quality traits at slaughter. From the H-sows, those with the intermediate (HI; n = 16) and those with the lowest (HL; n = 14) birth weight were selected. Selection from the L-sows included those with the intermediate (LI; n = 16) and those with the highest (LH; n = 15) birth weight, similar to that of the HL-piglets. Runt piglets with a birth weight of <0.8 kg were not considered for selection. Subsequently, BW and average daily gain (ADG) of all piglets were determined during lactation. From weaning until slaughter, the pigs selected were reared in group pens (eight pigs/pen) equipped with automatic feeder and individual pig recognition system (Schauer Maschinenfabrik GmbH. & Co KG, Prambachkirchen, Austria) as described previously (Bee et al., Reference Bee, Jacot, Guex and Herzog2004). Whenever possible, pigs of the same litter stayed in the same pen. Individual ad libitum intake of the starter (weaning to 28 kg BW), grower (28.1 to 63.5 kg BW) and finisher diets (63.6 kg BW until slaughter) was monitored and recorded by the control software (MLP, Schauer) linked to each feeder. The composition of these three diets is specified in Table 1. Pigs were weighed weekly. Growth performance data in the table are presented for the preweaning, starter and grower–finisher (28.1 kg to slaughter) periods.
Ingredients and nutrient composition of the experimental diets

1Supplied the following micronutrients per kilogram of diet: 20 000 IU of vitamin A, 200 IU of vitamin D3, 39 mg of vitamin E, 2.9 mg of riboflavin, 2.4 mg of vitamin B6, 0.01 mg of vitamin B12, 0.2 mg of vitamin K3, 10 mg of pantothenic acid, 1.4 mg of niacin, 0.48 mg of folic acid, 199 g of choline, 0.052 mg of biotin, 52 mg of Fe as FeSO4, 0.16 mg of I as Ca(IO3)2, 0.15 mg of Se as Na2Se, 5.5 mg of Cu as CuSO4, 81 mg of Zn as ZnO2, and 15 mg of Mn as MnO2.
2Pellet binder (Mikro-Technik, GmbH & Co. KG, Bürgstadt, Germany).
3Calculated as dry matter – total ash – crude fiber – CP – ether extract.
Slaughter procedure and carcass measurements
Pigs were slaughtered at 165 ± 1.5 days of age in the research station's abattoir. The last 15 h before slaughter, feed was withheld from the pigs. The animals were stunned in a CO2 stunner (87% CO2) for 100 s, immediately exsanguinated, scalded, mechanically de-haired, eviscerated and split along the mid-line within 30 min. Weights of hot carcass (total and left side), kidneys, spleen, liver, lung, heart and brain were assessed. Carcasses were then chilled at 2°C for 24 h. One day before post mortem, the total and left carcass side were weighed again to determine cold carcass weight and dissected into major primal cuts (loin, ham, shoulder and belly) and total lean meat was calculated as described previously (Bee et al., Reference Bee, Gebert and Messikommer2002). Back fat thickness was determined at the 10th rib level.
Meat quality measurements
Temperature and pH were measured 30 min and 24 h post mortem in the m. longissimus dorsi (LM; at the 10th rib level) and the dark portion of the m. semitendinosus (ST) using a pH meter (WTW pH 197-S; WTW, Weilheim, Germany) equipped with an insertion glass spearhead electrode (Metrohm, 6.0226.100) combined with a temperature probe (Pt 1000, Metrohm AG, Herisau, Switzerland). After the second assessment of pH and temperature, the entire ST was excised and weighed. Samples of the LM, harvested between the 10th and the 13th rib level, were cut into four 1.5 cm-thick slices free of subcutaneous adipose tissue and bone and labeled A, B, C and D. From the dark portion of the ST, two (E and F) longitudinal slices, weighing ∼70 g each, were prepared. The A, C and E slices were used to assess drip loss (48 h) using the plastic bag method by Honikel (Reference Honikel1998). After a 10 min bloom, the L* (lightness) values were determined on the B, D and F slices, using a spectrophotometer (model CM-2600d, Minolta, Dietikon, Switzerland). Three measurements on each sample were carried out and averaged. Afterwards, the B and D slices were weighed, vacuum-packed and stored at −20°C. Later the frozen samples were thawed for 24 h at 2°C and then weighed to determine thaw loss. After 1 h at room temperature, the slices were cooked on a preheated (190°C to 195°C) grill plate (Beer Grill AG, Zurich, Switzerland) to an internal temperature of 69°C recorded by a thermometer probe. The slices were cooked for 1.5 min on one side, then turned and cooked for 3.5 min, and finally 2 min on the initial side. Slices were reweighed to determine cooking loss. Approximately 2 h after cooking when meat samples reached room temperature, shear force was determined (five cores per sample) using a Stable Micro System TA.XT2 Texture Analyzer (Godalming, Surrey, UK) equipped with a 2.5-mm-thick Warner–Bratzler shear blade. Shear force values were expressed as the average of the five measurements.
Statistical analysis
Data were analyzed using the mixed procedure (SAS Inst. Inc., Cary, NC, USA). The statistical model used for analyzing the data from the reproductive performance of the sows and litter characteristics included the average weight of the litter (H- v. L-sows) as fixed effect and the sire nested within sows as random effect. Growth performance, carcass characteristics and meat quality traits of the pigs selected were analyzed with a model including birth weight group (HI, HL, LH, LI), gender and the two-way interactions. Sire nested within sow was included as a random effect. The pig was the experimental unit. Comparisons among least square means were made with the PDIFF statement using the Tukey–Kramer adjustment. Means were considered statistically different at P < 0.05 and referred to as tendencies at P < 0.10. The results are presented in the tables as least square means together with the pooled standard error.
Results
Reproductive performance of the sows
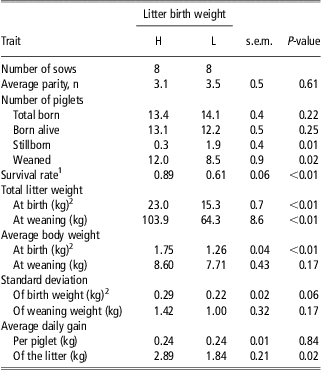
In both groups, the sows selected were on average in their third parity (Table 2). Litter size and number of piglets born alive were similar in the two groups, although the number of stillborns was greater (P = 0.01) in L- than in H-litters. Piglet survival rate during lactation was lower (P < 0.01) in L- compared with H-litters and, consequently, fewer (P = 0.02) piglets were weaned from L-litters. Despite a similar female-to-male ratio at birth in both experimental groups, L-sows weaned fewer (P < 0.07) female pigs (data not shown). As planned, the average litter birth weight of total piglets born alive clearly differed (P < 0.01), with the H-litters being 490 g heavier than the L-litters. Concomitantly, total litter weight at birth was lower (P < 0.01) for the L-litters than the H-litters. Compared with the H-litters, the L-litters birth weight of female pigs, but not male pigs, were less (P < 0.01) variable (data not shown). This resulted in an overall lower standard deviation in L-litters. Regardless of gender, ADG expressed per piglet was similar in both litter groups during lactation, but the high variation prevented the average weaning BW to be significantly different between groups. When calculated for the whole litter, total weaning weight and ADG of the litter were markedly lower (P ⩽ 0.02) in L- than in H-litters.
Reproductive performance of sows classified as having high (H > 1.7 kg)- or low (L < 1.3 kg)-average litter birth weight and litter sizes of between 10 and 15 total pigs born
1Calculated from birth to weaning.
2Calculations included piglets born alive only.
Birth weight and growth performance of the selected offspring
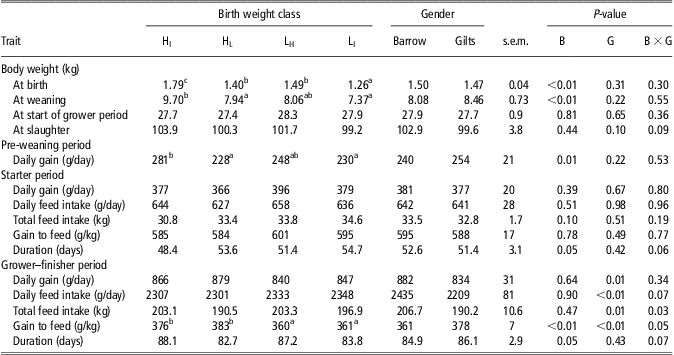
At birth, HL- and LH-piglets had similar average BW, whereas HI-piglets were 530 g heavier (P < 0.05) than LI-piglets (Table 3). Considering birth weight class within litter groups, HL-piglets were 390 g lighter (P < 0.05) than in HI-piglets, and LI-piglets were 230 g lighter (P < 0.05) than in LH-piglets. At weaning, the HI-piglets were still the heaviest group (P < 0.05 against HL and LI). In addition, the difference in BW was greater within the H- than within the L-litter piglet groups (HIv. HL = 1.76 kg and LHv. LI = 0.69 kg). This effect was related to the faster (P < 0.05) growth of HI- compared with HL-piglets during lactation. During the starter and grower–finisher periods, average daily feed intake (ADFI) and ADG were similar for all groups. Conversely, when comparing pigs born with similar birth weight but originating either from H- or L-litters (HLv. LH), the HL-pigs were more (P < 0.05) feed efficient in the grower–finisher period. At 165 days of age, the slaughter BW did not differ among groups. However, the time needed to reach the target BW in the grower–finisher period was shorter (P < 0.05) in HL- than in HI-pigs (with the L-litter pigs remaining intermediate) and appeared to be a compensation for the corresponding numerical longer starter period of the HL-pigs.
Effect of birth weight class and gender on growth performance during lactation, starter and growing–finishing periods of the selected pigletsFootnote 1
1 HI and HL = littermates with the intermediate (n = 16) and lowest (n = 14) birth weight within their litter, born from sows giving birth to litters classified as having high (>1.7 kg)-average litter birth weight; LH and LI = littermates with the greatest (n = 15) and intermediate (n = 16) birth weight within their litter born from sows giving birth to litters classified as having low (<1.3 kg)-average litter birth weight; n = 31 for barrow; n = 30 for gilts; B = birth weight class, G = gender.
a,b,c Least square means within a row for the main factor birth weight class without a common superscript differ (P < 0.05).
Gender differences were not observed in the starter period for any of the variables measured. Regardless of the birth weight class, gilts tended to have a lower (P = 0.10) slaughter weight at 165 days than barrows as a result of the lower (P ⩽ 0.01) ADG and ADFI in the grower–finisher period. Nevertheless, gilts were more feed efficient and total feed intake was proportionately lower in the same period than that of the barrows (P ⩽ 0.01 for each). Birth weight class × gender interactions (P ⩽ 0.05) were observed for the gain-to-feed ratio and total feed intake in the grower–finisher period. The HL-female pigs were the most feed efficient of all the other pig categories (Figure 1). In addition, compared with HL-barrows, HL-gilts consumed markedly less (P < 0.05) of the grower and finisher diets.
Effect of birth weight and gender on total feed intake and gain to feed ratio during the grower–finisher period. HI and HL = littermates with the intermediate and lowest birth weight within their litter, born from sows giving birth to litters classified as having high (>1.7 kg) average litter birth weight; LH and LI = littermates with the greatest and intermediate birth weight within their litter born from sows giving birth to litters classified as having low (<1.3 kg) average litter birth weight. a,b,cLeast square means without a common superscript differ (P < 0.05).
Carcass characteristics and morphometric data of the fattened offspring
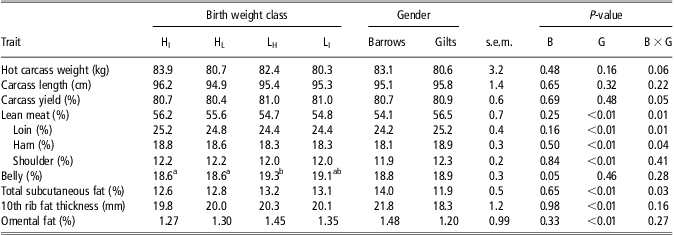
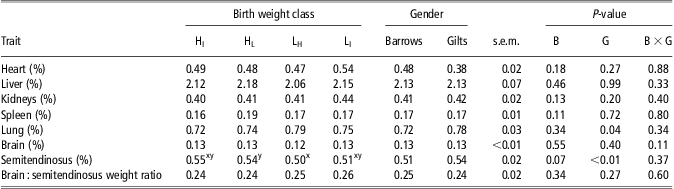
Birth weight had little impact on the carcass characteristics (Table 4). Belly percentage was lower (P < 0.05) in HL-pigs and HI-pigs compared with LH-pigs, with intermediate values for LI-pigs. As a result of the greater (P < 0.01) percentages of loin, ham and shoulder, and the lower (P < 0.01) percentages of omental and back fat, carcasses of gilts were leaner (P < 0.01) compared with those of barrows. However, the gender difference for lean meat, loin, ham and total subcutaneous fat percentages was mainly evident between female pigs and barrows born from H-litters, whereas LH- and LI-female pigs had similar percentages of loin, ham and subcutaneous fat than barrows (birth weight class × gender interaction; P ⩽ 0.03). Relative weight of internal organs and brain expressed as a percentage of hot carcass weight did not differ among birth weight classes and gender (Table 5). By contrast, the relative ST weight tended (P < 0.10) to be lower in LH- than in HL-pigs and was lower (P < 0.01) in barrows than gilts.
Effect of birth weight class and gender on carcass characteristicsFootnote 1
1 HI and HL = littermates with the intermediate (n = 16) and lowest (n = 14) birth weight within their litter, born from sows giving birth to litters classified as having high (>1.7 kg)-average litter birth weight; LH and LI = littermates with the greatest (n = 15) and intermediate (n = 16) birth weight within their litter, born from sows giving birth to litters classified as having low (<1.3 kg)-average litter birth weight; n = 31 for barrow; n = 30 for gilts; B = birth weight class, G = gender.
a,b Least square means within a row for the main factor birth weight class without a common superscript differ (P < 0.05).
Effect of birth weight class and gender on the relative weight of the internal organs, brain and semitendinosus muscleFootnote 1
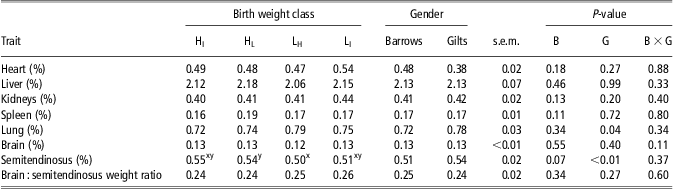
1 Relative weights of the organs and semitendinosus muscle are expressed as percentage of hot carcass weight. HI and HL = littermates with the intermediate (n = 16) and lowest (n = 14) birth weight within their litter, born from sows giving birth to litters classified as having high (>1.7 kg)-average litter birth weight; LH and LI = littermates with the greatest (n = 15) and intermediate (n = 16) birth weight within their litter born from sows giving birth to litters classified as having low (<1.3 kg)-average litter birth weight; n = 31 for barrow; n = 30 for gilts; B = birth weight class, G = gender.
x,y,a,b Least square means within a row for the main factor birth weight class without a common superscript differ (P < 0.10).
Quality of the meat from the fattened offspring
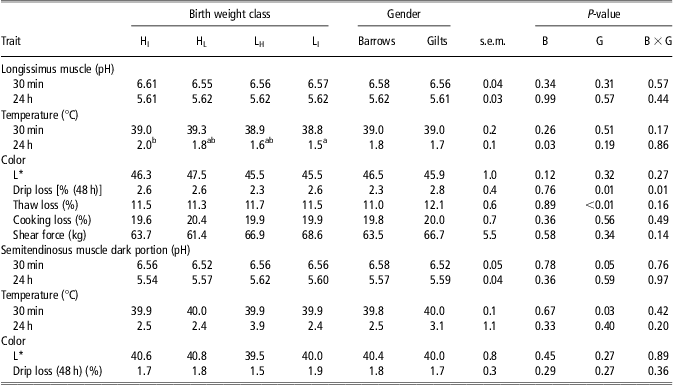
Birth weight class effects on the assessed meat quality traits were observed only for LM temperature at 24 h post mortem where temperature was lower (P < 0.05) in LI- than in HI-pigs, with intermediate values in LH-pigs and HL-pigs (Table 6). With respect to gender, pH and temperature at 30 min post mortem of the ST was greater (P ⩽ 0.05) in barrows than in gilts, whereas this was not the case in the LM. At 24 h post mortem, the pH and temperature of both muscles did not differ according to gender. Drip and thaw losses of the LM of barrows were lower (P ⩽ 0.01) than in the LM of the gilts.
Effect of birth weight class and gender on meat quality traits in slaughter pigsFootnote 1
1 HI and HL = littermates with the intermediate (n = 16) and lowest (n = 14) birth weight within their litter, born from sows giving birth to litters classified as having high (>1.7 kg)-average litter birth weight; LH and LI = littermates with the greatest (n = 15) and intermediate (n = 16) birth weight within their litter born from sows giving birth to litters classified as having low (<1.3 kg)-average litter birth weight; n = 31 for barrow; n = 30 for gilts; B = birth weight class, G = gender.
a,b Lleast square means within a row for the main factor birth weight class without a common superscript differ (P < 0.05).
Discussion
Sow performance in relation to average litter birth weight
A greater incidence of low birth weight piglets has been associated with increased litter size, the latter being the consequence of intensive breeding efforts in the last few decades with the objective to enhance the prolificacy of dams and ultimately improve reproduction efficiency (Milligan et al., Reference Milligan, Fraser and Kramer2002; Quiniou et al., Reference Quiniou, Dagorn and Gaudré2002; Quesnel et al., Reference Quesnel, Brossard, Valancogne and Quiniou2008).
In the current study, the difference in average litter birth weight between L- and H-litters was ∼500 g. In contrast to other studies (e.g., Bérard et al., Reference Bérard, Kreuzer and Bee2008), this magnitude of difference in birth weight was unrelated to the number of total born. Nevertheless, in the present study, the standard deviation of within-litter birth weight tended to be lower in L- than in H-litters. Foxcroft et al. (Reference Foxcroft, Bee, Dixon, Hahn, Harding, Patterson, Putman, Sarmento, Smit, Tse and Town2007) explained this phenomenon as a consequence of prenatal losses of weaker and smaller embryos and fetuses, thereby reducing intra-litter variability in birth weight. Another striking difference between the two litter birth weight groups was the greater proportion of stillborn in L- (13%) compared with H-litters (2%), which, except for the fact that in the present case it was unrelated to litter size, matches results of earlier studies (Leenhouwers et al., Reference Leenhouwers, van der Lende and Knol1999; Milligan et al., Reference Milligan, Fraser and Kramer2002; Quiniou et al., Reference Quiniou, Dagorn and Gaudré2002). As observed by Leenhouwers et al. (Reference Leenhouwers, van der Lende and Knol1999), a low average birth weight is associated with a greater pre-weaning mortality, which was more than three times greater in L- than in H-litters (39% v. 11%, respectively). The 33% difference between L- and H-litters in total litter weight at birth increased to 38% at weaning. In accordance with Bérard and Bee (Reference Bérard and Bee2010), ADG during lactation was independent of birth weight. Our findings are in contrast to results reported by Quiniou et al. (Reference Quiniou, Dagorn and Gaudré2002) showing that during lactation heavier piglets grow faster than lighter piglets. These authors assumed that heavier piglets have a greater ability to occupy the best-performing teats, to stimulate and to drain them, thereby inducing a larger milk flow. However, because of the greater number of stillborn and greater mortality rate in L- than in H-litters, and as no cross-fostering was performed in the current study, competition among littermates for the teats was markedly reduced after the first week of lactation. Thus, growth of L-offspring was not hindered by lacking nutrient supply.
Growth performance as affected by birth weight class and gender
The pigs selected at weaning to evaluate growth performance, carcass and meat quality traits mirrored the selection criteria of the experimental design, as birth weights of LI- and HI-pigs were close to the average birth weight of the respective litters and LH- and HL-pigs had a similar birth weight. Therefore, based on the results of previous studies reporting a close relationship between birth weight and early postnatal growth (Gondret et al., Reference Gondret, Lefaucheur, Juin, Louveau and Lebret2006; Bérard et al., Reference Bérard, Kreuzer and Bee2010), the ranking of BW at weaning could have been expected to remain similar for the four groups as at birth (HI>LH = HL>LI). In fact, this relationship was confirmed in the H-litters where growth rate and weaning weight depended on birth weight. By contrast in the L-litters, LI-pigs reached comparable weaning weights as their heavier littermates (LH). A likely explanation for the similar growth rate might be found in the greater mortality rate in L-litters that entailed less competition for teats and therefore nutrient supply from sow milk, and thus might not have limited growth of lighter and usually less vital pigs. Along the same line of explanation, it was unexpected to observe that LH-pigs did not translate the greater nutrient availability into greater growth rates, as their ADG was comparable to the one of HL-pigs.
Consistent with results of previous studies (Gondret et al., Reference Gondret, Lefaucheur, Louveau, Lebret, Pichodo and Le Cozler2005; Bérard et al., Reference Bérard, Kreuzer and Bee2008; Bérard et al., Reference Bérard, Kreuzer and Bee2010), pigs born with a lower birth weight displayed catch-up growth, because differences in BW between the four experimental groups gradually disappeared after weaning. To compensate for the 2.33 kg lower weaning weight, it took the lightest pigs (LI) on average 6.3 days longer than the heaviest pigs (HI) to reach the beginning of the grower period, which was defined to start at an average BW of 27 kg. This helps explaining the greater total intake of starter diet in LI- compared with HI-pigs, as neither ADG nor ADFI gains to feed ratio differed between the birth weight groups. In the grower–finisher period, feed efficiency was lower in L- than in H-offspring owing to the numerically lower ADG and greater ADFI. Consistent with the study by Bérard et al. (Reference Bérard, Kreuzer and Bee2010), this effect was more distinct in female pigs, implying that under ad libitum feed supply, especially female pigs, born from low average litter birth weight sows, will perform less efficiently.
Except for the relative ST weights, which tended to be lower in LH- than in HL-pigs and were lower in barrows than gilts, neither birth weight nor gender affected relative weights of internal organs and brain. This was surprising in view of the fact that using a similar experimental design, Pardo et al. (Reference Pardo, Kreuzer and Bee2010) reported a lower relative brain weight (expressed relative to the birth weight) in HI- than in LI-newborns and lower in HL- than in LH-newborns. This had let the authors conclude that those lighter piglets had some characteristics associated with growth retardation as supported by other studies (Bauer et al., Reference Bauer, Walter, Brust, Fuchtner and Zwiener2003; Town et al., Reference Town, Patterson, Pereira, Gourley and Foxcroft2005; Vallet and Freking, Reference Vallet and Freking2006). Furthermore, it was shown that an impaired development of organs such as the kidneys, heart and liver can still be observed in low birth weight compared with high birth weight pigs when they reach the slaughter weight (Bérard et al., Reference Bérard, Kreuzer and Bee2008; Rehfeldt et al., Reference Rehfeldt, Tuchscherer, Hartung and Kuhn2008; Nissen and Oksbjerg, Reference Nissen and Oksbjerg2011). Therefore, based on the findings on organ weight and carcass composition, it is difficult to assess whether, or to which extent, offspring from L-sows had been subjected to intrauterine growth retardation.
Carcass and meat quality as affected by birth weight class and gender
The data published on the impact of birth weight on carcass characteristics are inconsistent owing to differences in applied feeding strategies, rearing conditions or range of birth weight used in the various studies. For instance, carcasses of low birth weight compared with high birth weight pigs were fatter at slaughter if pigs were reared in individual pens and had ad libitum access to the diet (Gondret et al., Reference Gondret, Lefaucheur, Juin, Louveau and Lebret2006). By contrast, carcass composition was similar when low birth weight and high birth weight pigs penned in groups had restricted access to the feed (Gondret et al., Reference Gondret, Lefaucheur, Louveau, Lebret, Pichodo and Le Cozler2005). Covering a wide birth weight range of up to 850 g, data of various studies reported no relationship between birth weight and lean meat percentage (Gondret et al., Reference Gondret, Lefaucheur, Louveau, Lebret, Pichodo and Le Cozler2005; Bérard et al., Reference Bérard, Kreuzer and Bee2008; Beaulieu et al., Reference Beaulieu, Aalhus, Williams and Patience2010). By contrast, when differences in birth weight were ∼900 g, Rehfeldt and Kuhn (Reference Rehfeldt and Kuhn2006) found a tendency toward leaner carcasses in low birth weight (0.94 kg) compared with high (1.80 kg) birth weight pigs slaughtered at the same age. However, in a similar study by the same authors, carcass leanness did not differ when birth weight differences were <400 g (1.39 v. 1.80 kg or 1.37 v. 1.67 kg) (Rehfeldt and Kuhn, Reference Rehfeldt and Kuhn2006; Rehfeldt et al., Reference Rehfeldt, Tuchscherer, Hartung and Kuhn2008). Thus, it appears that the ratio of adipose and muscle tissue deposition rate is affected only in littermates with very low birth weight, which might explain the lack of effect on carcass characteristics in the current experiment with a difference in average birth weight of up to 530 g (LI- v. HI-pigs). Furthermore, it has to be kept in mind that, in contrast to all of the aforementioned studies where pigs with extremely high or low birth weight were compared, LI-pigs were in the intermediate birth weight range within their litters and were 320 and 180 g heavier than the piglets in the studies by Rehfeldt and Kuhn (Reference Rehfeldt and Kuhn2006) and Rehfeldt et al. (Reference Rehfeldt, Tuchscherer, Hartung and Kuhn2008), respectively. Nevertheless, there was one exception. Belly percentage, which is a cut with a great amount of intermuscular fat, was greater in LH- compared with HL-pigs and HI-pigs, suggesting that the impaired feed efficiency of the LH-pigs in the grower–finisher period affected this pork cut.
Usually when female pigs and barrows have ad libitum access to the grower–finisher diets, carcasses of female pigs are leaner at slaughter (Ellis et al., Reference Ellis, Webb, Avery and Brown1996; Rehfeldt et al., Reference Rehfeldt, Tuchscherer, Hartung and Kuhn2008; Bérard et al., Reference Bérard, Kreuzer and Bee2010). This difference was noticeable between gilts and barrows born from the H-litters, whereas percentages of lean meat, loin, ham, subcutaneous and back fat were similar in gilts and barrows of the LH-group and LI-group. In addition, these findings match the similar feed efficiency found in the grower–finisher period in the L-litters. Results of other studies also suggested that low birth weight has stronger effects on carcass composition in female pigs compared with male pigs (Poore and Fowden, Reference Poore and Fowden2004; Gondret et al., Reference Gondret, Lefaucheur, Juin, Louveau and Lebret2006; Bérard et al., Reference Bérard, Kreuzer and Bee2010).
Effects of birth weight or gender on technological traits of the LM and dark portion of the ST were marginal, which matches results of previous studies (Nissen et al., Reference Nissen, Jorgensen and Oksbjerg2004; Bérard et al., Reference Bérard, Kreuzer and Bee2008; Rehfeldt et al., Reference Rehfeldt, Tuchscherer, Hartung and Kuhn2008; Beaulieu et al., Reference Beaulieu, Aalhus, Williams and Patience2010).
In conclusion, this study confirms the occurrence of negative effects on viability and pre-weaning performance of piglets born from litters with a low average weight probably as a result of low gestation efficiency. This gets obvious by the increased number of stillborns and a greater pre-weaning mortality of progeny. Therefore, the number of piglets weaned was reduced, which adversely affected sow performance. Contrary to expectations, low birth weight did not impair postnatal growth of their individuals and, thus fattening performance and the initial variability in weight observed at birth in these litters of normal size gradually disappeared after weaning. There was also no differences in the brain : muscle ratio at slaughter making assumptions about the presence or absence of intrauterine crowding as a reason for low average birth weight inconclusive. Within the litters, gender variability caused more effects on postnatal growth in the L-litters, particularly in the female pigs, than in the H-litters. Further studies have to identify the reasons for the differences in the efficiency in sows with apparently normal litter size and the gender-dependence adverse effects on performance of the offspring of low birth weight litters.
Acknowledgments
The authors thank Guy Maïkoff and his team for taking care of the animals, and Dr Paolo Silacci and his team for the help during sample collection and muscle analysis. This study was supported by the Fondation Sur-la-Croix (Basel, Switzerland).