





Highlights
1. Lexical competition impairs non-native naming and increases cognitive control demands.
2. Trait and state control differentially shape Stroop facilitation versus interference.
3. Higher proficiency and balanced language use predict better naming performance.
4. Proficient multilinguals dynamically recruit control networks under high competition.
5. Language-specific and domain-general regions jointly support conflict resolution.
1. Introduction
Language production broadly refers to expressing thoughts through spoken or written language (Roger et al., Reference Roger, Banjac, Thiebaut de Schotten and Baciu2022), which relies on complex cognitive and neural mechanisms (Fedorenko & Thompson-Schill, Reference Fedorenko and Thompson-Schill2014; Laganaro et al., Reference Laganaro, Tzieropoulos, Frauenfelder and Zesiger2015; Zhang et al., Reference Zhang, Eppes, Beatty-Martínez, Navarro-Torres and Diaz2018). Multilinguals often manage several languages, which creates greater competition and places higher demands on cognitive control than in monolingual speakers (Green, Reference Green1998; Kroll et al., Reference Kroll, Bobb and Wodniecka2006). However, it remains unclear how multilingual experience shapes the influence of cognitive control on language production, both behaviorally and neurally—particularly in the more demanding context of non-native language use. This study investigates how multilingual experience, indexed by proficiency and usage, modulates the role of cognitive control traits and states in non-native language production.
Language production transforms thoughts into speech through coordinated processes (Crowther & Martin, Reference Crowther and Martin2014; Nozari, Reference Nozari2025; Ye & Zhou, Reference Ye and Zhou2009), including conceptual and lexical retrieval, articulatory planning, attentional control and verbal monitoring (Badre & Wagner, Reference Badre and Wagner2007; Thompson-Schill et al., Reference Thompson-Schill, Bedny and Goldberg2005; Zhang et al., Reference Zhang, Eppes, Beatty-Martínez, Navarro-Torres and Diaz2018). When producing a word, selecting one target among several semantically similar alternatives increases lexical competition (Britt et al., Reference Britt, Ferrara and Mirman2016; Maxfield, Reference Maxfield2020; Moss et al., Reference Moss, Abdallah, Fletcher, Bright, Pilgrim, Acres and Tyler2005). For example, a picture of “a long, soft seat” may activate both “sofa” and “couch,” delaying naming and increasing errors compared with dominant representations like “banana” (Apfelbaum et al., Reference Apfelbaum, Goodwin, Blomquist and McMurray2023; Zhang & Samuel, Reference Zhang and Samuel2018). Lexical competition is often indexed by name agreement (Alario et al., Reference Alario, Ferrand, Laganaro, New, Frauenfelder and Segui2004). Higher name agreement reflects a single common label, whereas lower agreement indicates multiple acceptable names (Brodeur et al., Reference Brodeur, Guerard and Bouras2014; Snodgrass & Vanderwart, Reference Snodgrass and Vanderwart1980). Lower name agreement heightens competition, highlighting the role of cognitive control in resolving lexical conflict and supporting fluent production (Alario et al., Reference Alario, Ferrand, Laganaro, New, Frauenfelder and Segui2004; Swingley & Aslin, Reference Swingley and Aslin2007).
During production, multilinguals face both within-language lexical competition and cross-language lexical interference, often from their more proficient or frequently used language (Marian & Spivey, Reference Marian and Spivey2003; Sarrett et al., Reference Sarrett, Shea and McMurray2022; Zhang et al., Reference Zhang, Zheng and Wu2025b). Effective non-native language production thus depends strongly on cognitive control. Neuroimaging studies show that non-native production engages not only core language regions but also domain-general regions. For instance, the left inferior frontal gyrus (LIFG) extending to bilateral frontal cortex are involved in response inhibition and interference resolution (Badre, Reference Badre2008; Hampshire et al., Reference Hampshire, Chamberlain, Monti, Duncan and Owen2010; Novick et al., Reference Novick, Trueswell and Thompson-Schill2005; Swick et al., Reference Swick, Ashley and Turken2008), playing a vital role in managing lexical competition and resolving conflict during production (Abutalebi & Green, Reference Abutalebi and Green2008; Calabria et al., Reference Calabria, Jefferies, Sala, Morenas-Rodríguez, Illán-Gala, Montal, Fortea, Lleó and Costa2021; De Bleser et al., Reference De Bleser, Dupont, Postler, Bormans, Speelman, Mortelmans and Debrock2003; Liu et al., Reference Liu, de Bruin, Jiao, Li and Wang2021). Domain-general control regions also contribute to the monitoring and regulation of language output, as evidenced by increased activation in the left dorsolateral prefrontal cortex (DLPFC) when speakers must resolve competition among multiple activated spoken responses (Abutalebi & Green, Reference Abutalebi and Green2016; Collette et al., Reference Collette, Olivier, Van der Linden, Laureys, Delfiore, Luxen and Salmon2005; Videsott et al., Reference Videsott, Herrnberger, Hoenig, Schilly, Grothe, Wiater, Spitzer and Kiefer2010).
Importantly, cognitive control can be considered at both trait and state levels. Cognitive control traits refer to relatively stable individual differences in the ability to maintain task goals, inhibit irrelevant information, monitor conflict and resolve interference (Allen & Potkay, Reference Allen and Potkay1981; Salig et al., Reference Salig, Valdes Kroff, Slevc and Novick2021; Steyer et al., Reference Steyer, Mayer, Geiser and Cole2015). In contrast, cognitive control states reflect transient adjustments in control that occur in response to immediate task demands, such as increased control following a conflict trial (Maki-Marttunen et al., Reference Maki-Marttunen, Hagen and Espeseth2019; Menon & D’Esposito, Reference Menon and D’Esposito2022), thereby influencing competition resolution in language processing (Hsu & Novick, Reference Hsu and Novick2016; Ovans et al., Reference Ovans, Hsu, Bell-Souder, Gilley, Novick and Kim2022). This distinction is theoretically important for language production because trait and state control may operate on different timescales and support different aspects of lexical competition resolution. Control traits shape a speaker’s general efficiency in managing lexical competition, whereas control states may support moment-to-moment adjustments when conflict is temporarily increased (Carter et al., Reference Carter, DeLuca, Segaert, Mazaheri and Krott2023). Thus, separating these two dimensions allows us to examine whether language production depends primarily on stable control capacity, transient conflict-driven adjustment, or both. Previous research shows that both cognitive control traits and transient control states modulate performance in native language production (Zhang et al., Reference Zhang, Kang, Zhong, Yu, Ip and Zhang2025a). Given the greater control demands involved in non-native production, these effects may be even stronger, particularly under conditions of high lexical competition.
Earlier research on multilingualism and cognitive control often compared bilinguals with monolinguals. However, multilingual experience varies greatly across individuals, a pattern increasingly acknowledged in recent years (Gullifer et al., Reference Gullifer, Chai, Whitford, Pivneva, Baum, Klein and Titone2018; Gullifer & Titone, Reference Gullifer and Titone2020; Gullifer & Titone, Reference Gullifer and Titone2021a). This experience can be characterized by ability-based and usage-based dimensions, both of which may influence how cognitive control contributes to language production (Kheder & Kaan, Reference Kheder and Kaan2021). From an ability-based perspective, studies have reported that higher non-native language proficiency is positively associated with better cognitive control and production performance (Abutalebi et al., Reference Abutalebi, Della Rosa, Ding, Weekes, Costa and Green2013; Abutalebi & Green, Reference Abutalebi and Green2007; Green & Abutalebi, Reference Green and Abutalebi2013; Poarch & van Hell, Reference Poarch and van Hell2012; Vega-Mendoza et al., Reference Vega-Mendoza, West, Sorace and Bak2015). For example, compared with lower-proficiency multilinguals, those with higher non-native language proficiency show superior performance on reactive and proactive inhibitory control tasks, reflected in reduced inhibitory costs regardless of the acquisition age (Costa et al., Reference Costa, Colomé, Gómez and SebastiÁN-GallÉS200 Reference Abutalebi and Green3; Yow & Li, Reference Yow and Li2015). Higher-proficiency multilinguals also engage monitoring mechanisms more effectively (Bialystok et al., Reference Bialystok, Craik, Grady, Chau, Ishii, Gunji and Pantev2005; Costa et al., Reference Costa, Colomé, Gómez and SebastiÁN-GallÉS200 Reference Abutalebi and Green3), supporting efficient task execution and goal maintenance. Neuroimaging studies have shown that increased non-native language proficiency reduces the need for controlled processing (i.e., competition resolution becomes more automatic) and is associated with decreased activation in the LIFG and anterior cingulate cortex (Abutalebi & Green, Reference Abutalebi and Green2007; Briellmann et al., Reference Briellmann, Saling, Connell, Waites, Abbott and Jackson2004; Tatsuno & Sakai, Reference Tatsuno and Sakai2005).
From a usage-based perspective, multilinguals differ in how often they use languages within the same context (Green & Abutalebi, Reference Green and Abutalebi2013; Wagner et al., Reference Wagner, Bekas and Bialystok2023), placing varying demands on cognitive control. Language entropy has been proposed and validated as a measure of diversity and balance in language use (Gullifer & Titone, Reference Gullifer and Titone2020). Individuals with higher entropy tend to use multiple languages more evenly across contexts, requiring greater engagement of control resources (Gullifer & Titone, Reference Gullifer and Titone2021a,Reference Gullifer and Titoneb; Sulpizio et al., Reference Sulpizio, Del Maschio, Del Mauro, Fedeli and Abutalebi2020). Neuroimaging studies further support this, showing stronger connectivity between the bilateral putamen and anterior cingulate cortex (ACC)—regions linked to non-native language speech production and executive function (Gullifer et al., Reference Gullifer, Chai, Whitford, Pivneva, Baum, Klein and Titone2018; Li et al., Reference Li, Zatorre and Du2021; Salig et al., Reference Salig, Valdes Kroff, Slevc and Novick2021). Additionally, lifelong demands for conflict monitoring and resolution in multilinguals may lead to more efficient or automatic control engagement (Folstein & Van Petten, Reference Folstein and Van Petten2008; Markiewicz et al., Reference Markiewicz, Mazaheri and Krott2023). This has been reflected in a stronger N2 component, which signals monitoring demands (Kousaie & Phillips, Reference Kousaie and Phillips2012; Markiewicz et al., Reference Markiewicz, Mazaheri and Krott2023), and reduced activation of executive-control regions (e.g., superior, middle, and inferior frontal gyri) that support interference control and response selection. Together, these findings suggest that specific aspects of multilingual experience shape individual cognitive and neural profiles, which in turn may modulate non-native language production.
Despite evidence linking cognitive control to non-native language production, few studies have examined how individual differences in control ability and transient control states interact with non-native proficiency and multilingual usage. To address this gap, the present study investigates how variations in multilingual experience—specifically non-native language proficiency and diversity of language use—shape the behavioral and neural dynamics of non-native word production through cognitive control mechanisms. Participants completed a picture naming task in their non-native language English in the MRI scanner, with some pictures designed to induce higher lexical competition through lower name agreement. Cognitive control states were manipulated using a preceding Stroop trial (conflict versus non-conflict), while individual control traits were assessed with three established cognitive control tasks. Multilingual language background was indexed by non-native language proficiency and usage patterns. We predicted that higher proficiency and greater language use diversity would enhance non-native language production performance and reduce neural effort, particularly during high lexical competition. Critically, we further expected multilingual experience to modulate the relationship between cognitive control and non-native language production. Rather than treating cognitive control as a unitary construct, we examined both trait-level and state-level control to determine whether multilingual experience shapes the contribution of stable control capacities, transient control adjustments, or both.
2. Methods
2.1. Participants
Forty native Cantonese speakers living in Macau (14 males, mean age = 23 years, range = 18–32 years) were tested (demographic information is reported in Table 1). All participants reported normal or corrected-to-normal vision and were right-handed as determined by the Edinburgh Handedness Inventory (Oldfield, Reference Oldfield1971). No participants reported a history of neurological or psychiatric disorders. All participants spoke English as their non-native language and demonstrated a high level of English proficiency through the updated Vocabulary Levels Test (Webb et al., Reference Webb, Sasao and Ballance2017), with vocabulary test scores all above 70, corresponding approximately to an International English Language Testing System (IELTS) score of 6. Informed consent was obtained before the experiment, ensuring that participants were fully aware of the study’s purpose, procedures, potential risks, and benefits. The authors confirm that all procedures contributing to this work comply with the ethical standards of the relevant national and institutional committees on human experimentation and with the Declaration of Helsinki of 1975, as revised in 2008. The Research Ethics Committee of the University of Macau (protocol code BSERE22-APP001-ICI, approved on March 17, 2022) approved all the guidelines and study protocols.
Participants’ demographic characteristics and neuropsychological testing scores

Table 1. Long description
The table is organized into three columns: Measure, Mean, and S D.
Demographic information:
* N: 40.
* Age in years: Mean 22.93, S D 2.74.
* Education in years: Mean 16.44, S D 2.31.
* Gender Female forward slash Male: 26 forward slash 14.
Language measures:
* Language entropy: Mean 0.85, S D 0.32.
* Verbal fluency English (Animal, Correct token): Mean 18.53, S D 4.30.
Cognitive control traits measures:
* A X minus C P T: A Y minus A X R T in milliseconds: Mean 74.40, S D 40.10.
* Simon effect (Incongruent minus Congruent) in milliseconds: Mean 36.38, S D 23.27.
* Flanker effect (Incongruent minus Congruent) in milliseconds: Mean 53.75, S D 22.34.
2.2. Stimuli and procedure
Neuropsychological testing was conducted prior to the MRI session. During this session, participants completed the Language History Questionnaire (LHQ3; Li et al., Reference Li, Zhang, Yu and Zhao2020), from which language entropy was calculated to quantify individual differences in language experience; a categorical verbal fluency (VF) task to assess English proficiency; and three cognitive tasks designed to evaluate their cognitive control traits, including the AX version of the Continuous Performance task (AX-CPT), Simon task and Flanker task.
2.2.1. Language History Questionnaire
Participants first completed the Language History Questionnaire (LHQ3; Li et al., Reference Li, Zhang, Yu and Zhao2020), capturing multilingual language usage. Across 17 communicative contexts, participants reported the time spent on each language (e.g., on social media, reading, writing or speaking with different people) and the frequency of language activities on a 7-point scale (including various types of self-directed activities). Based on these data, language entropy was calculated, quantifying individuals’ multilingual experience by estimating the diversity of language use across social contexts (Gullifer et al., Reference Gullifer, Chai, Whitford, Pivneva, Baum, Klein and Titone2018; Gullifer & Titone, Reference Gullifer and Titone2020, Reference Gullifer and Titone2021a,Reference Gullifer and Titoneb). This approach is grounded in Shannon entropy (Shannon, Reference Shannon1948), a classic measure of information uncertainty and diversity. Language entropy for each context was calculated using the following formula:
$ H=-{\sum}_{i=1}^n{P}_i{\mathit{\log}}_2\left({P}_i\right), $
 where
$ n $
 represents the total number of possible languages within a given context, and
$ {P}_i $
 is the proportion of use of a specific language in that context. The calculations were performed using the Language Entropy package (Gullifer & Titone, Reference Gullifer, Chai, Whitford, Pivneva, Baum, Klein and Titone2018) in the R environment (R Core Team, 2024). The mean entropy across all contextual domains was then computed for each participant. Lower entropy values indicate more unbalanced and less diverse language use, while higher entropy values indicate more balanced and varied language use across different contexts.
2.2.2. English verbal fluency
Language proficiency was assessed using a categorical VF task, where participants generated as many English animal names as possible within 1 min (Felicetti, Reference Felicetti201 Reference Abutalebi, Della Rosa, Ding, Weekes, Costa and Green2; Patterson, Reference Patterson, Kreutzer, DeLuca and Caplan2011). A higher number of correct responses indicates better VF performance, therefore, greater English proficiency, whereas fewer correct responses suggest a more limited vocabulary and relatively lower proficiency.
2.2.3. Cognitive control tasks
To evaluate cognitive control traits, three cognitive tasks were administered in the current study. Details regarding these tasks have been previously reported in Zhang et al. (Reference Zhang, Kang, Zhong, Yu, Ip and Zhang2025a). Briefly, in the AX version of the Continuous Performance Task (Braver et al., Reference Braver, Barch, Keys, Carter, Cohen, Kaye, Janowsky, Taylor, Yesavage, Mumenthaler, Jagust and Reed2001), participants were instructed to make a Yes response when an A cue was followed by an X probe (AX trials), and a No response otherwise (AY, BX, BY trials) within each sequence of five letters. In the Simon task (Simon & Wolf, Reference Simon and Wolf1963), participants were instructed to press the right key for a blue square and the left key for a red square, irrespective of its location from either congruent trials (e.g., a blue square on the right side requiring a right key response) or incongruent trials (e.g., a blue square on the left side requiring a right key response). Additionally, in the Flanker task (Eriksen & Eriksen, Reference Eriksen and Eriksen1974), participants were instructed to respond to the direction of a central arrow while ignoring surrounding flankers from congruent trials (e.g., the central target and the surrounding arrows pointing in the same direction), incongruent trials (e.g., the central target and the surrounding arrows pointing in the different direction) and neutral trials (e.g., the surrounding stimuli are diamond shapes instead of arrows). To assemble a universal indicator of cognitive control traits for each participant, task-specific cognitive control index was first calculated (i.e., response time difference for AY – AX in AX-CPT, incongruent – congruent in the Simon task, and incongruent – congruent in the Flanker task; Table 1), then each index was standardized by being converted to a Z score and summed to a composite Z score. Finally, the composite Z scores were reverse coded into a cognitive control trait score, so that a higher trait score indicates better cognitive control ability.
2.2.4. In-scanner word production task
Following the neuropsychological session, participants performed an English word production task that incorporated a Stroop manipulation into picture naming in the MRI scanner (Figure 1), to examine the effect of cognitive control states on word production. The task involved six color words (i.e., blue, green, red, brown, orange, and yellow) displayed in one of three ink colors (i.e., blue, green, and red). Trials were either congruent, in which the word and ink color matched (Figure 1A,C), or incongruent, where they did not match (Figure 1B,D). Incongruent Stroop trials elicited representational conflict between the prepotent response and the task-relevant color naming, increasing cognitive control demands compared to congruent trials. By presenting Stroop trials before the picture naming trials, cognitive control states were modulated (i.e., conflict trials requiring higher cognitive control states versus non-conflict trials requiring lower cognitive control states).
In-scanner Stroop-embedded picture naming task examples.
Note: In each pair, the Stroop trial, then the picture was presented sequentially on a white background for 1.5 s each, separated by a blank screen for 0.5 s. A variable duration of fixation between pairs (ISI, range = 2.5–16.5 s, average ISI = 4.1 s) was used. Stroop trials in A and C are green printed in green; in B and D are orange printed in green; pictures in A and B have lower lexical competition (H-index: 0 ± 0); pictures in C and D have higher lexical competition (H-index: 1.04 ± 0.42).

Figure 1. Long description
The diagram consists of four panels, A, B, C, and D, each showing a sequence of three screens on a white background. Each sequence follows a timeline from left to right.
* Panel A (Non-conflict and Lower lexical competition): Starts with a fixation cross for 2.5 to 16.5 s, followed by a 0.5 s blank screen. Next is a Stroop trial showing the word ‘green’ printed in green ink for 1.5 s, followed by a 0.5 s blank screen. It ends with a picture of a banana for 1.5 s.
* Panel B (Conflict and Lower lexical competition): Follows the same timing as A. The Stroop trial shows the word ‘orange’ printed in green ink. It ends with a picture of a banana.
* Panel C (Non-conflict and Higher lexical competition): Follows the same timing as A. The Stroop trial shows the word ‘green’ printed in green ink. It ends with a picture of a green sofa.
* Panel D (Conflict and Higher lexical competition): Follows the same timing as A. The Stroop trial shows the word ‘orange’ printed in green ink. It ends with a picture of a green sofa.
Below each sequence, a horizontal arrow points to the right, indicating the progression of time in seconds (s).
Pictures for the naming task were selected from the MultiPic norm (Duñabeitia et al., Reference Duñabeitia, Crepaldi, Meyer, New, Pliatsikas, Smolka and Brysbaert2018). The norm consists of 750 colored line drawings illustrating concrete concepts. An independent group of 28 healthy, native Cantonese speakers normed these stimuli. They were asked to provide the most appropriate name in English. The name agreement of each picture was then calculated using the H-index (Brodeur et al., Reference Brodeur, Guerard and Bouras2014). Among these pictures, 100 items with lower name agreement were selected to elicit higher lexical competition, while 100 items with higher name agreement were selected to elicit lower lexical competition.
To this end, a 2 (Conflict status: conflict versus non-conflict) × 2 (Lexical competition: higher versus lower) within-subject design was formed. The final set included 50 pictures for each of the four conditions. The name agreement in the higher lexical competition conditions was significantly lower than that in the lower lexical competition conditions (p < 0.001). Stimuli across conditions were statistically matched on familiarity, target word length, visual complexity and word frequency (ps > 0.1). An additional 50 pictures were selected for the control condition. Unlike the critical conditions that contain only Stroop-Picture pairs, the control condition includes Stroop-Stroop, Picture-Picture, and Picture-Stroop trials to prevent participants from predicting upcoming trials or task types. In each pair of all conditions, both stimuli were presented on a white background for 1.5 s, separated by a blank screen for 0.5 s (Figure 1). A variable inter-stimulus interval after each pair (ISI, range = 2.5–6.5 s, average ISI = 4.1 s) was used, generated by the optseq2 program, as jittered presentations can optimize the hemodynamic response (Dale, Reference Dale1999).
Before scanning, participants practiced the task while minimizing head movement in an MRI simulator. After practice, participants completed five runs of the picture naming task in the scanner, each containing 10 stimulus pairs from every condition. Picture stimuli were not repeated across conditions. Before each picture, participants were presented with a Stroop trial, in which they needed to say the ink color of a color word in English (e.g., say “green” for the word orange printed in green ink). During the picture trial, participants were presented with pictures and instructed to overtly name the picture in English as quickly and accurately as possible. The overt verbal responses during the scan were recorded and online filtered using an MR-compatible fiber optic microphone system (Optoacoustics Ltd., Or-Yehuda, Israel).
2.3. Acquisition of MRI data
MRI scanning was completed using a 3T Siemens Prisma MRI scanner equipped with a 32-channel head coil. A sagittal T1-weighted localizer was first acquired to define a volume for subsequent data collection, higher-order shimming, and alignment to the AC-PC line (i.e., Anterior and Posterior Commissure). Then T1-weighted anatomical images were collected using the magnetization-prepared rapid acquisition gradient echo (MP-RAGE) sequence (repetition time [TR] = 2300 ms; echo time [TE] = 2.28 ms; flip angle = 8°; field of view [FOV] = 256 mm2; voxel size = 1.0 × 1.0 × 1.0 mm3; phase encode direction: anterior to posterior; fat saturation = off; duration = 5 minutes and 21 seconds).
After the structural images were obtained, participants underwent task runs in the scanner. Task-based functional images sensitive to BOLD contrast were acquired using an echo-planar imaging (EPI) sequence (TR = 2000 ms; TE = 25.0 ms; flip angle = 90°; FOV = 240 mm2; voxel size = 3.0 × 3.0 × 4.0 mm3; 33 contiguous slices; phase encode direction: anterior to posterior; fat saturation = on; duration = 6 minutes and 36 seconds per run; 5 runs).
A field map sequence was also acquired using an echo sequence (TR = 436.0 ms; TE1 = 4.92 ms; TE2 = 7.38 ms; flip angle = 60°; FOV = 240 mm2; voxel size = 3.0 × 3.0 × 4.0 mm3; 33 contiguous slices; phase encoding direction: anterior to posterior, fat saturation = off; duration = 1 minute and 12 seconds), generating two magnitude images and one phase image.
2.4. Behavioral data coding
Responses for the Stroop-embedded picture naming task were coded based on the recordings during the scan. For each run, the participant’s verbal responses were transcribed precisely, and the accuracy of each response was assessed. For Stroop stimuli, responses were coded as correct only when participants accurately named the ink color. All other responses, including omissions, were coded as incorrect. For picture stimuli, responses were coded as correct when the spoken responses were exactly the same as the target word (e.g., “mailbox” for mailbox) or they described the same concept (e.g., “letterbox” for mailbox). If the produced word was inconsistent with the picture concept (e.g., “door” for mailbox) or not aligned with specific concepts (e.g., “box” for mailbox), the responses were coded as incorrect. Both stimuli in a Stroop-Picture pair had to be correctly responded to for the trial to be considered correct. Reaction times (RTs) for all trials were calculated using customized PRAAT scripts, by calculating the interval between the onset of the stimulus and the initiation of the verbal response. After calculation, RTs were trimmed first. Only reaction times from the correctly responded trials and within the 2.5 standard deviation of each participant’s mean were included in the analysis.
2.5. MRI data preprocessing
Prior to data processing, data quality was evaluated using the fBIRN QA tool (Glover et al., Reference Glover, Mueller, Turner, van Erp, Liu, Greve, Voyvodic, Rasmussen, Brown, Keator, Calhoun, Lee, Ford, Mathalon, Diaz, O’Leary, Gadde, Preda, Lim and Potkin2012), assessing the mean signal fluctuation-to-noise ratio (SFNR), the number of potentially clipped voxels, and variation per slice. Subsequently, the anatomical and functional images were visually checked for artifacts and signal dropout. The non-brain portions were identified and removed from structural images using Optimized Brain Extraction for Pathological Brains (Lutkenhoff et al., Reference Lutkenhoff, Rosenberg, Chiang, Zhang, Pickard, Owen and Monti2014). Preprocessing and statistical analyses were conducted using the FSL FEAT (fMRI expert analysis tool) version 6.0 (Smith et al., Reference Smith, Jenkinson, Woolrich, Beckmann, Behrens, Johansen-Berg, Bannister, De Luca, Drobnjak, Flitney, Niazy, Saunders, Vickers, Zhang, De Stefano, Brady and Matthews2004; Woolrich et al., Reference Woolrich, Behrens, Beckmann, Jenkinson and Smith2004). Preprocessing included motion correction with MCFLIRT (Jenkinson et al., Reference Jenkinson, Bannister, Brady and Smith2002), B0 fieldmap-based unwarping, slice timing correction, spatial smoothing with a 5 mm FWHM Gaussian kernel, highpass temporal filtering, coregistration and normalization. All processed datasets were aligned to each participant’s anatomical image and then to the MNI152 standard space. For modeling the event-related BOLD signal, a double-gamma hemodynamic response function was used, including only correct trials in the analyses.
2.6. Behavioral and fMRI data analysis
RTs and the number of correct responses were analyzed using a mixed-effects regression conducted in the R statistical environment (R version 4.4.2; R Core Team, Reference Team2020). To examine how multilingual experience (i.e., non-native language proficiency and language use experience) influences the interaction between cognitive control and non-native language production, particularly under higher lexical competition demands, the model included cognitive control states (conflict versus non-conflict), cognitive control traits, lexical competition (higher versus lower), VF, language entropy, and their interactions as predictors. The final model can be specified as:
$ CorrectResponses/ RT= State\times Competition\times Trait\times VF+ State\times Competition\times Trait\times Entropy+\left(1+ State+ Competition\;\right|\; Subject\Big)+\left(1+ Trait+ VF+ Entropy\;|\; Probe\_ Stimulus\right) $
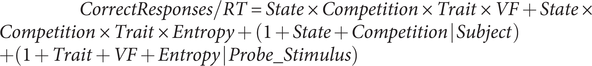 . All continuous variables were standardized.
For the basic fMRI activation analysis, events were time-locked to the onset of each Stroop trial and each picture, enabling precise measurement of brain activity associated with word production. For the preprocessed fMRI data, first-level analyses were performed on the individual runs for each participant. Higher-level group analyses were then conducted to combine first-level results across runs and then across subjects. Although the activation associated with Stroop processing was modeled, we primarily focused on brain activation associated with picture naming. Specifically, the contrast of lexical competition reflected by name agreement (higher versus lower) was modeled to explore the BOLD response during picture naming using a general linear model in FSL. This contrast was masked with regions activated in the higher lexical competition conditions to ensure that the reported regions were functionally meaningful.
In addition to the whole-brain analysis of picture-evoked fMRI activation, we examined the regional fluctuations in neural activation associated with the picture-naming task, and the effects of other control and multilingual variables. For this, we used a Region-Of-Interest (ROI) approach. Specifically, ROIs were extracted based on clusters showing stronger activation for pictures with higher lexical competition compared to those with lower competition. After extracting the maximum activation value of each ROI during picture naming, the same models as the behavioral analyses were conducted. To avoid circular inference, we did not interpret or report statistical tests of the main effect of lexical competition within these ROIs. Instead, the ROI analyses focused on interaction effects involving lexical competition, cognitive control traits, cognitive control states, language proficiency, and language entropy. To control for false discovery rate (FDR) in multiple comparisons, we applied the Benjamini–Hochberg (BH) procedure (Benjamini & Hochberg, Reference Benjamini and Hochberg1995) across ROIs. Adjusted p-values (q) were computed based on the rank of each original p-value and were then compared with a predefined significance threshold (
$ \alpha =0.05 $
 ).
3. Results
3.1. Behavioral results
To examine how cognitive control influences word production and how this relationship is modulated by multilingual experience, we conducted mixed-effects regression analyses on both the number of correct responses and reaction times (RTs). The models included lexical competition, cognitive control states, cognitive control traits, English VF, language entropy and their interactions as predictors. The analysis was conducted with one model for each performance index, but different sets of effects are reported in separate sections below for clarity.
3.1.1. Effects of cognitive control states and traits
For correct responses, the main effect of lexical competition (Figure 2A; β = −0.54, SE = 0.24, z = −2.30, p = 0.03) was significant, indicating that pictures with lower lexical competition were responded to more accurately than those with higher competition. The interaction between lexical competition and cognitive control traits was only nearly significant (p = 0.06). The main effects of cognitive control states and traits, the two-way interactions (states × lexical competition and states × traits), and the three-way interaction (states × traits × lexical competition) were all not significant (ps > 0.1).
Behavioral effects of cognitive control states, traits, and lexical competition on picture naming.
Note: A shows a significant main effect of lexical competition on accuracy, B shows a significant main effect of lexical competition on response times, C shows a significant interaction between cognitive control states and traits on response times. Error bars represent a mean ± standard error (SE). Lower trait values indicate poorer inhibitory control, while higher trait values indicate better inhibitory control.

Figure 2. Long description
A three-panel figure labeled A, B, and C.
Panel A is a box plot. The y-axis is Accuracy ranging from 0.4 to 0.9. The x-axis is Lexical Competition with two categories: Higher and Lower. The Higher category has a median accuracy of approximately 0.62, while the Lower category has a higher median accuracy of approximately 0.68.
Panel B is a box plot. The y-axis is Response Time in m s ranging from 1000 to 1600. The x-axis is Lexical Competition with two categories: Higher and Lower. The Higher category shows a higher median response time of approximately 1300 m s, while the Lower category shows a lower median response time of approximately 1180 m s.
Panel C is a line graph. The y-axis is Response Time in m s ranging from 1100 to 1400. The x-axis is Cognitive Control Traits ranging from negative 3 to positive 2. Two lines represent Conflict Status: a dark line for Conflict and a light blue line for Non-conflict. Both lines show a downward linear trend as traits increase. The Conflict line starts higher at approximately 1390 m s and ends lower at approximately 1130 m s. The Non-conflict line starts at approximately 1340 m s and ends at approximately 1170 m s. The lines intersect at a trait value of approximately 0.5. Shaded areas around the lines represent S E.
For RTs, the main effect of lexical competition (Figure 2B; β = 100.38, SE = 25.65, t (181.78) = 3.91, p < 0.001) was significant, indicating that pictures with lower lexical competition were responded to with faster speed than those with higher competition. Additionally, the interaction between cognitive control states and traits was significant (Figure 2C; β = −22.93, SE = 9.24, t (1180.15) = −2.48, p = 0.01), suggesting that individuals with higher control ability showed a facilitation effect from the proceeding Stroop conflict trials on subsequent picture naming. On the other hand, individuals with lower control ability showed an interference effect on the proceeding Stroop conflict trials on subsequent picture naming. Apart from the reported effects, the main effects of cognitive control states and traits, the two-way interactions (state × lexical competition; trait × lexical competition), and the three-way interaction (state × trait × lexical competition) were all not significant (ps > 0.1). Overall, these results demonstrate a strong interference effect from lexical competition, a conditional influence of cognitive control states on picture naming depending on individual cognitive control traits.
3.1.2. Effects of multilingual experience
For correct responses, the main effect of VF was significant (β = 0.56, SE = 0.11, z = 5.25, p < 0.001), indicating that participants with higher English proficiency tended to name the pictures more accurately (Figure 3A). Furthermore, the interaction between language entropy and cognitive control states was significant (β = 0.20, SE = 0.06, z = 3.09, p = 0.002), showing that individuals with more balanced language use were better able to adapt to the conflict resolution, leading to improved word production performance after Stroop conflict trials (Figure 3B).
Behavioral effects of cognitive control states, traits, lexical competition, verbal fluency, and language entropy on picture naming.
Note: A shows significant main effect of verbal fluency on accuracy, B shows a significant interaction between cognitive control states and language entropy on accuracy, C shows a significant interaction between lexical competition and verbal fluency on response times, D shows a nearly significant interaction between cognitive control states, traits, and verbal fluency (VF) on response times, E shows a nearly significant main effect of language entropy on response times. Lower trait score indicates poorer inhibitory control, while higher trait score indicates better inhibitory control.

Figure 3. Long description
Panel A is a scatter plot with a linear regression line. The x-axis is V F ranging from minus 2 to 3 and the y-axis is Accuracy from 0.5 to 0.9. The data shows a positive linear correlation between V F and Accuracy.
Panel B is a line graph with shaded error regions. The x-axis is Entropy from minus 2 to 2 and the y-axis is Accuracy from 0.55 to 0.75. A black line for Conflict shows a steep positive slope, while a blue line for Non-conflict remains relatively flat.
Panel C is a line graph with shaded error regions. The x-axis is Verbal Fluency from minus 2 to 3 and the y-axis is Response Time in m s from 1000 to 1400. A solid purple line for Higher Lexical Competition and a dashed purple line for Lower Lexical Competition both show a downward trend, with the dashed line having a steeper negative slope.
Panel D contains two side-by-side line graphs. The x-axis is Cognitive Control Traits from minus 3 to 2 and the y-axis is Response Time in m s from 1100 to 1500. The left plot for High underscore V F shows black and blue lines with moderate negative slopes. The right plot for Low underscore V F shows a much steeper negative slope for the black Conflict line compared to the blue Non-conflict line.
Panel E is a scatter plot with a linear regression line. The x-axis is Entropy from minus 2 to 2 and the y-axis is Response Time in m s from 1000 to 1600. The data shows a slight negative linear trend.
For RTs, the main effect of VF was significant (β = −63.76, SE = 28.02, t (41.08) = −2.28, p = 0.03), such that participants with higher English proficiency showed faster picture naming responses (Figure 3C). Additionally, the interaction between VF and lexical competition was significant (β = 32.21, SE = 13.64, t (55.97) = 2.36, p = 0.04). Specifically, individuals with higher English proficiency showed a larger lexical competition effect, manifested as a greater facilitation on pictures with lower lexical competition (Figure 3C). Furthermore, the three-way interaction between VF, cognitive control states and traits was marginally significant (β = 16.28, SE = 9.13, t (1137.91) = 1.78, p = 0.07). Specifically, as reported earlier, individuals with stronger control abilities (reflected by a higher trait score) showed greater adaptability to name pictures after conflict Stroop trials, and this effect is more pronounced among lower-proficiency individuals (Figure 3D). Moreover, the main effect of language entropy also tended toward significance (β = −51.56, SE = 27.41, t (39.95) = −1.88, p = 0.07), such that more balanced language use was associated with faster picture naming (Figure 3E).
In summary, these findings demonstrate a variable influence of cognitive control states and traits on word production performance, modulated by multilingual language experience.
3.2. fMRI results
3.2.1. Basic activation to lexical competition
Compared to pictures with lower lexical competition, those with higher lexical competition elicited stronger activation in the left hemisphere regions, including the inferior frontal gyrus (IFG), extending to the superior and middle frontal gyri (SFG, MFG), frontal pole and precentral gyrus, as well as the bilateral lateral occipital cortex (Figure 4A, Table 2).
(A) Brain regions exhibiting significantly stronger activation in response to higher lexical competition pictures compared to lower lexical competition pictures. Slides displayed ranged from z = -10, to z = 60; the activation Z value ranges from 3.1 to 6.2. (B)–(F) Among all regions shown in Panel A, these areas exhibited significant modulation by cognitive control and multilingual experience after correction for multiple comparisons: (B) and (C) frontal pole, (D) insula, (E) pars triangularis of the IFG and (F) pars opercularis of the IFG.
Note: Con = Conflict; Non = Non-conflict; IFG = Inferior Frontal Gyrus. All reported in MNI space coordinate.

Figure 4. Long description
Panel A displays two lateral views of a brain and eight axial slices labeled z equals minus 10 to z equals 60. Red and yellow heat maps indicate activation intensity from 3.1 to 6.2. Panels B through F show neural intensity graphs for specific regions.
Panel B: A point-and-line graph for the Frontal Pole. The y-axis is Frontal Pole Intensity (1.5 to 2.5). The x-axis shows Conflict Status (Con- and Non-). Higher lexical competition (solid line) consistently shows higher intensity than lower competition (dashed line) across Higher and Lower Entropy groups.
Panel C: A linear regression for the Frontal Pole. The y-axis is intensity (1 to 3). The x-axis is Cognitive Control Traits (minus 3 to 2). In the Higher Entropy group, intensity increases with traits; in the Lower Entropy group, the trend is slightly negative.
Panel D: A linear regression for the Insula. The y-axis is Insula Intensity (1.0 to 2.5). The x-axis is Verbal Fluency (minus 2 to 3). Higher lexical competition shows a positive slope, while lower competition shows a negative slope.
Panel E: A linear regression for the I F G tri (pars triangularis). The y-axis is intensity (2 to 4). The x-axis is Cognitive Control Traits. Both Higher and Lower Entropy groups show positive slopes, with higher lexical competition maintaining a higher intercept.
Panel F: A linear regression for the I F G op (pars opercularis). The y-axis is intensity (2 to 5). The x-axis is Verbal Fluency. Both lexical competition levels show a positive correlation with fluency, with higher competition exhibiting a steeper upward trend.
3.2.2. Effects of multilingual experience and cognitive control on production
To explore the dynamic recruitment of neural resources in regions exhibiting stronger activation for pictures with higher lexical competition than for pictures with lower lexical competition, the same linear mixed-effects regression as in the behavioral analyses was conducted on each ROI’s maximum activation intensity (eight ROIs reported in Table 2 except occipital clusters). Significance was assessed using the Benjamini–Hochberg procedure (q < 0.05).
Brain activation to lexical competition

Table 2. Long description
The table lists brain regions activated during lexical competition (Higher > Lower) in M N I space. Columns include Hemisphere, Voxels, Coordinates (x, y, z), and Z value.
* Insula (left): 137 voxels, coordinates (-30, 24, 4), Z value 4.33.
* Middle frontal gyrus (left): 2090 voxels, coordinates (-46, 14, 34), Z value 5.71. Sub-regions include:
- Frontal pole: (-42, 46, 0), Z value 4.29.
- Inferior frontal gyrus, Pars opercularis: (-48, 16, 28), Z value 5.08.
- Inferior frontal gyrus, Pars triangularis: (-46, 32, 13), Z value 3.69.
- Precentral gyrus: (-48, 8, 29), Z value 3.62.
* Superior frontal gyrus (left): 1279 voxels, coordinates (-4, 20, 54), Z value 6.30. Includes Paracingulate gyrus at (-4, 20, 48), Z value 6.22.
* Lateral occipital cortex (left): 1060 voxels, coordinates (-36, -84, 24), Z value 4.57. Includes Occipital pole at (-16, -98, 2), Z value 4.07.
* Lateral occipital cortex (right): 349 voxels, coordinates (38, -82, 18), Z value 5.01.
Note: All reported in MNI space coordinate.
In the frontal pole, the interaction between cognitive control states and lexical competition was moderated by language entropy (Figure 4B, β −36.64, SE = 8.61, t (40) = −4.25, p < 0.001, q = 0.001). Specifically, among individuals with higher language entropy, adaptation from conflict Stroop trials improved the implementation of control during picture naming, allowing them to manage higher competition pictures with fewer additional resources than in non-conflict conditions. Furthermore, the interaction between lexical competition and cognitive control traits also varied as a function of language entropy (Figure 4C, β −24.96, SE = 7.52, t (40) = −3.32, p = 0.002, q = 0.019). The involvement of the frontal pole in resolving lexical competition was more pronounced in individuals with higher cognitive control trait scores among those with higher language entropy. In contrast, for individuals with lower entropy, greater cognitive control traits were associated with reduced engagement of the frontal pole during lexical selection.
In the insula (Figure 4D), we observed a significant interaction between lexical competition and VF (β = 18.52, SE = 5.44, t (40) = 3.40, p = 0.002, q = 0.015). This finding suggests that individuals with greater VF recruited fewer neural resources from insula when naming items with lower lexical competition, but engaged additional insula resources when naming items with higher lexical competition. In contrast, individuals with lower VF showed no significant difference in insula activation across levels of lexical competition.
In the IFG pars triangularis (Figure 4E), the competition-by-trait interaction also varied as a function of language entropy (β = −23.27, SE = 77.74, t (40) = −3.01, p = 0.005, q = 0.041). Specifically, individuals with higher cognitive control traits and language entropy showed greater IFG involvement in resolving lexical competition, mirroring the pattern observed in the frontal pole. On the other hand, for individuals with lower entropy, better cognitive control ability was associated with reduced IFG engagement during lower lexical competition but increased engagement during higher lexical competition.
Similarly, in the IFG pars opercularis (Figure 4F), we also observed a significant interaction between lexical competition and VF (β = 25.60, SE = 7.10, t (56.02) = 3.60, p < 0.001, q = 0.007), indicating that with greater VF, individuals needed to recruit additional neural resources from the opercularis part of the IFG to support picture naming—particularly for pictures with higher lexical competition.
Together, these findings suggest that trait- and state-level cognitive control, together with multilingual experience, shaped the recruitment of frontal control regions under high lexical competition. Individuals with stronger control abilities and richer language experience show greater insula and frontal engagement when competition is higher.
4. Effects of stroop interference and lexical competition on production
To examine whether the Stroop-induced control states and lexical competition in the word-production task rely on shared control resources, we conducted a Pearson correlation analysis. Control efficiency was indexed by each task’s interference effect: the Stroop effect was calculated as the RT difference between conflict and non-conflict trials, and the lexical competition effect was calculated as the RT difference between higher- and lower-competition pictures. A significant positive correlation was found between the Stroop effect and lexical competition effect (Figure 5, r (38) = 0.42, p = 0.008), suggesting that individuals with greater Stroop interference also showed larger lexical competition costs, indicating partially shared control mechanisms across tasks.
Behavioral effects of Stroop and lexical competition on picture naming.

Figure 5. Long description
A scatter plot with the x-axis labeled Stroop Effect R T ranging from 0 to 400 and the y-axis labeled Lexical Competition Effect R T ranging from 0 to 300. In the top-left corner, statistical values are listed as R equals 0.42 and p equals 0.0077. The data consists of approximately 40 teal circular data points scattered across the plot. A dark blue linear regression line starts at approximately y equals 50 on the left and rises to y equals 200 on the right, indicating a positive linear increase. The line is surrounded by a light gray shaded area representing the confidence interval, which widens as it moves toward the right side of the graph. Most data points are clustered between 50 and 200 on the x-axis and 0 and 200 on the y-axis, with one notable outlier at the top center near x equals 250 and y equals 350.
5. Discussion and conclusion
This study investigated how cognitive control influences non-native language production in multilingual individuals, with a particular focus on control mechanisms interacting with varying language proficiency and usage. Our results revealed a reliable interference effect of lexical competition behaviorally and neurally, which was more pronounced in individuals with higher non-native language proficiency. Moreover, participants with richer multilingual experience demonstrated more efficient word production, as evidenced by faster naming and more adaptive neural recruitment. The contribution of cognitive control traits and states to non-native word production was further modulated by multilingual experience. Below, we discuss these findings in detail.
First of all, this study demonstrated a robust lexical competition effect both behaviorally and neurally. Pictures with higher lexical competition elicited lower naming accuracy, longer response times, and greater activation in language and control regions, including the left frontal pole and superior, middle and inferior frontal gyri. The involvement of the left IFG, MFG, and SFG aligns with prior findings on increased engagement during low name agreement processing in native language production (Cheng et al., Reference Cheng, Schafer and Akyurek2010; Zhang et al., Reference Zhang, Kang, Zhong, Yu, Ip and Zhang2025a). On the other hand, the activation of the frontal pole appears uniquely tied to the lexical competition effect in non-native language production, suggesting its critical role in managing increased control demands during production. This region is widely recognized as a hub for domain-general executive control, supporting processes such as goal maintenance, conflict monitoring and inhibition (Badre & Nee, Reference Badre and Nee2018; Chayer & Freedman, Reference Chayer and Freedman2001; Schall et al., Reference Schall, Stuphorn and Brown2002). Its engagement in non-native production likely reflects the need to suppress automatic native-language responses and overcome perseverative tendencies from prior tasks to maintain task goals. Previous studies have also reported recruitment of domain-general regions—including the frontal pole and dorsolateral prefrontal cortex—during non-native language tasks, underscoring the reliance on broader control networks beyond core language areas (Gullifer et al., Reference Gullifer, Chai, Whitford, Pivneva, Baum, Klein and Titone2018; Videsott et al., Reference Videsott, Herrnberger, Hoenig, Schilly, Grothe, Wiater, Spitzer and Kiefer2010). Additionally, processing pictures with lower name agreement further amplifies frontal pole involvement, highlighting its contribution to managing uncertainty and resolving lexical competition.
Beyond frontal regions, our study also revealed stronger activation in the left insula and precentral gyrus during higher lexical competition, a pattern that appears specific to non-native language production, compared with previous studies investigating native language production using similar paradigms (Zhang et al., Reference Zhang, Kang, Zhong, Yu, Ip and Zhang2025a). The insula cortex, widely recognized for its involvement in speech motor control and domain-general cognitive processes (Calabria et al., Reference Calabria, Costa, Green and Abutalebi2018; Menon, Reference Menon and Grafman2025; Wang et al., Reference Wang, Ke, Zhang, Zhou, Li and Yang2020), likely supports articulatory planning and conflict resolution in non-native contexts. Similarly, the precentral gyrus, traditionally associated with motor planning, may facilitate the execution of complex articulatory sequences required for accurate naming (Geschwind, Reference Geschwind1970; Silva et al., Reference Silva, Liu, Zhao, Levy, Scott and Chang2022; Turker et al., Reference Turker, Kuhnke, Eickhoff, Caspers and Hartwigsen2023). Prior fMRI evidence also reported that the left precentral gyrus contributes to semantic and lexical processing in non-native language tasks (Van de Putte et al., Reference Van de Putte, De Baene, Brass and Duyck2017), underscoring the integration of motor and control systems in bilingual word production. Collectively, these findings indicate that lexical competition in non-native language production engages a distributed network that includes both language-specific control regions and domain-general control areas.
Beyond identifying behavioral and neural mechanisms of lexical competition in non-native word production, this study also examined how cognitive control states and traits influence this process. First, a significant positive correlation was observed between the Stroop effect and lexical competition effect, supporting the involvement of overlapping neural systems in cognitive control across tasks. This finding is consistent with domain-generality accounts (Nozari, Reference Nozari2025), which propose shared control mechanisms for different domains. These accounts further predict that manipulating control in one domain would influence performance in another. Behaviorally, our findings revealed a shift between cross-task facilitation and interference in non-native language production, depending on individual cognitive control traits. Specifically, individuals with better control ability named pictures faster after Stroop conflict trials than after Stroop non-conflict trials, whereas those with worse control ability showed slower naming following Stroop conflict trials. This pattern indicates distinct modulation of conflict effects across Stroop-picture pairs based on trait-level control. Previous studies using similar paradigms have reported general cross-task conflict adaptation in language comprehension without considering individual differences (Hsu & Novick, Reference Hsu and Novick2016). Our results suggest that individuals with stronger cognitive control abilities, characterized by more efficient and automatic control processes (Marton, Reference Marton2024), adapted more effectively to transient control states, resulting in facilitation in naming. Importantly, this facilitation occurs in overall naming performance rather than in resolving lexical competition. In contrast, individuals with weaker control abilities may experience cross-task interference in partial overlap tasks (e.g., Stroop and picture naming), likely due to increased cognitive demands and competition for limited control resources.
In addition to the effects of cognitive control traits and states, multilingual experience—indexed by VF (proficiency) and language entropy (usage)—was associated with more effective word production, particularly through better resolution of lexical competition with distinct patterns of neural activation. First, we found that multilinguals with higher proficiency and more frequent use of multiple languages named pictures in English faster and more accurately. This advantage likely reflects more efficient word retrieval supported by their extensive experience with the non-native language English (Abutalebi, Reference Abutalebi2008; Padilla & Chen, Reference Padilla, Chen, Padilla and Chen2025; Videsott et al., Reference Videsott, Herrnberger, Hoenig, Schilly, Grothe, Wiater, Spitzer and Kiefer2010). Interestingly, for individuals with higher English proficiency, the lexical competition effect was more pronounced, likely due to a larger vocabulary that introduces greater competition among alternative responses. Consistent with these behavioral findings, individuals with higher proficiency showed increased recruitment of left insula and opercular regions of the IFG to resolve greater lexical competition (Ardila et al., Reference Ardila, Bernal and Rosselli2014; Friederici et al., Reference Friederici, Bahlmann, Heim, Schubotz and Anwander2006; Medaglia et al., Reference Medaglia, Harvey, Kelkar, Zimmerman, Mass, Bassett and Hamilton2021; Oh et al., Reference Oh, Duerden and Pang2014; Sharp et al., Reference Sharp, Scott, Cutler and Wise2005). Importantly, this stronger lexical competition effect does not contradict their overall better naming performance; rather, both patterns stem from the same underlying factor—greater proficiency expands lexical options, which enhances naming speed overall but also amplifies competition when multiple alternatives are activated.
Furthermore, language proficiency significantly modulated the interaction between cognitive control traits and states on production. To recap briefly, individuals with stronger control abilities adapted better after conflict trials and showed cross-task facilitation, whereas those with weaker control abilities tended to experience interference from the previous Stroop conflict trials. This interaction was primarily driven by individuals with lower language proficiency, highlighting strategic differences in how speakers with varying experience allocate control resources during production (Figure 3D). For these individuals, limited vocabulary knowledge increases lexical retrieval difficulty and amplifies overall cognitive demands (Videsott et al., Reference Videsott, Herrnberger, Hoenig, Schilly, Grothe, Wiater, Spitzer and Kiefer2010), especially for those with weaker control abilities. Because they lack well-established lexical representations in the non-native language, word selection tends to be slower and more effortful. Consequently, they are more vulnerable to cross-task modulation (Hsu & Novick, Reference Hsu and Novick2016) during non-native word production, making interference or adaptation effects from previous trials more pronounced.
In addition to ability-based findings, our results showed that multilingual experience modulated the cross-task effects from cognitive control state to non-native language production, similar to the interaction observed between control traits and states. Specifically, individuals with mixed and balanced language use—often associated with more efficient and automatic inhibition control (Kałamała et al., Reference Kałamała, Walther, Zhang, Diaz, Senderecka and Wodniecka2022; Yow & Li, Reference Yow and Li2015)—adapted more effectively to transient control states and exhibited conflict facilitation on overall naming (Figure 3B). In contrast, those with less diverse language use were more likely to experience interference in Stroop-embedded picture naming tasks, likely due to reduced availability of cognitive control resources following conflict trials. Neurally, the lexical competition effect in left frontal pole was modulated by an interaction between cognitive control state and multilingual experience, highlighting its role in integrating language experience with cognitive control processes. Specifically, reduced recruitment of the frontal pole after Stroop conflict trials suggests a lower demand for control resources during subsequent picture naming. This facilitation effect was further amplified in individuals with more extensive multilingual experience, likely reflecting greater cognitive control capacity and supporting conflict adaptation at the behavioral level.
Furthermore, both the left frontal pole and the triangular part of the inferior frontal gyrus (IFG) were sensitive to the modulation of multilingual experience on the interaction between cognitive control traits and lexical competition. Among individuals with more extensive multilingual experience, Stroop trials appeared to consume fewer neural resources (Gullifer & Titone, Reference Gullifer and Titone2021a,Reference Gullifer and Titoneb; Wagner et al., Reference Wagner, Bekas and Bialystok2023), allowing greater allocation of neural resources to resolve lexical competition during word production. This was reflected in a larger lexical competition effect in frontal pole and IFG activation among individuals with higher control trait scores. On the other hand, individuals with less multilingual experience may have limited cognitive control, constraining the neural resources available for picture naming across conditions. This results in a smaller neural difference between high- and low-competition items in these regions. However, multilinguals with less extensive language experience but higher control traits relied more on the left IFG (triangular portion) for high-competition items—similar to those with greater multilingual experience—while showing less engagement of the frontal pole. This pattern underscores the priority of recruiting IFG for language-specific control and competition resolution over domain-general resources (Indefrey & Levelt, Reference Indefrey and Levelt2000; Kim et al., Reference Kim, Relkin, Lee and Hirsch1997; Vingerhoets et al., Reference Vingerhoets, Van Borsel, Tesink, Van Den Noort, Deblaere, Seurinck, Vandemaele and Achten2003).
The study provides direct evidence that multilingual experience is related to non-native language production patterns. However, some findings are constrained by the nature of our measures and warrant further investigation. In the present study, non-native language proficiency was indexed by VF total score, which has been widely used in bilingual and second-language research as an indicator of lexical retrieval efficiency and productive language ability (Gullifer et al., Reference Gullifer, Kousaie, Gilbert, Grant, Giroud, Coulter, Klein, Baum, Phillips and Titone2021; Luo et al., Reference Luo, Luk and Bialystok2010). In our sample, VF performance was significantly correlated with self-reported English proficiency, averaged across listening, speaking, reading, and writing (p < .001), suggesting that it provides an objective measure that complements self-report. Nevertheless, VF is not a pure measure of language proficiency because performance also depends on executive processes related to controlled search, monitoring, and response selection. Future research should use multiple proficiency measures to better separate language ability from domain-general control processes.
Overall, this study examines the relationships between multilingual experience and cognitive control in non-native language production. Behavioral performance and neural activity revealed a strong and stable lexical competition effect during naming tasks, highlighting the engagement of cognitive control resources. Individuals with superior cognitive control benefited more from cross-task adaptation from conflict resolution to naming. More experienced multilinguals demonstrated better naming performance but also exhibited stronger lexical competition effects, underscoring the complexity of managing larger lexicons. The involvement of cognitive control was particularly pronounced in multilingual individuals with richer language experience, reflected in greater activation of both language-specific and domain-general brain regions. These findings emphasize the importance of considering individual multilingual experiences when investigating cognitive control in non-native language production.
Data availability statement
Data and analysis scripts are available at https://osf.io/mpfvt/.
Acknowledgments
This project was funded by the National Natural Science Foundation of China [32200845], the Science and Technology Development Fund, Macao S.A.R [FDCT, 0153/2022/A], and the Multi-Year Research Grant [MYRG-GRG2025-00227-ICI] from the University of Macau to Haoyun Zhang. We thank Jiaxi Yang for data collection, Xinzhu Liu, Ziye Zhang, Xiaobin Lu, and Xingying Li for MRI recording transcription. We thank the staff at the Centre for Cognitive and Brain Sciences (CCBS) at the University of Macau, where the study was conducted, for their support. The authors declare no conflicts of interest.
Author contribution
Conceptualization: S.Z., H.Z.; Data Curation: S.Z.; Formal analysis: S.Z.; Funding acquisition: H.Z.; Investigation: S.Z., H.Z.; Methodology: S.Z., H.Z.; Project administration: H.Z.; Resources: S.Z., H.Z.; Supervision: H.Z.; Visualization: S.Z.; Writing – Original Draft: S.Z.; Writing – Review & Editing: S.Z., H.Z.
Funding statement
This project was funded by the National Natural Science Foundation of China [32200845], the Science and Technology Development Fund, Macao S.A.R [FDCT, 0153/2022/A], and the Multi-Year Research Grant [MYRG-GRG2025–00227-ICI] from the University of Macau to Haoyun Zhang.
Conflicts of interest
The authors declare no conflicts of interest.


 Open access

