


INTRODUCTION
There is considerable interest in the ecological, immunological and evolutionary consequences of parasitic co-infection. This growing interest has resulted in a rapid expansion in the number of field and laboratory experiments aimed at determining whether, and how, different parasite species interact within the host and how the host responds, immunologically or otherwise, to such co-infection (Pedersen and Fenton, Reference Pedersen and Fenton2007). Central to many of these empirical studies is the role that host immune responses may play in mediating interactions between co-infecting parasites and determining the duration and severity of infections (e.g. Cox, Reference Cox2001; Graham et al. Reference Graham, Cattadori, Lloyd-Smith, Ferrari and Bjornstad2007; Page, Scott and Manabe, Reference Page, Scott and Manabe2006). In particular, the role of the T helper cell responses and their associated cytokines to individual and co-infecting parasites has been well elucidated under laboratory conditions. These studies show that vertebrate hosts typically respond to microparasites (such as viruses, bacteria and protozoa) with T helper 1 (Th1)-biased immune responses, whereas macroparasites (such as helminths) tend to elicit Th2-biased responses (Abbas, Murphy and Sher, Reference Abbas, Murphy and Sher1996). Importantly, the two types of immune responses act via very different effector mechanisms and thus fight different types of infections (Abbas et al. Reference Abbas, Murphy and Sher1996). For example, Th1 responses can promote phagocytosis of infected cells by macrophages, whereas Th2 responses can lead to the production of large volumes of mucus and other effector mechanisms that help to purge the gut of helminths.
The inter-relationships of these responses can be complex, depending, for example, on the locality of each infection (Lamb et al. Reference Lamb, Graham, Le Geoff and Allen2005), the host's nutritional status (Koski and Scott, Reference Koski and Scott2001), and interactions with alternative T helper cell types that control the magnitude of both Th1 and Th2 responses (e.g. regulatory T cells; Mills, Reference Mills2004). However, as a broad generalization, empirical evidence suggests that Th1 and Th2 immune responses are antagonistic (Abbas et al. Reference Abbas, Murphy and Sher1996), such that hosts cannot simultaneously mount strong responses of both types in one anatomical location. This mutual inhibition is observed even in the absence of nutritional limitation – indeed, most laboratory animals are fed ad lib – and may instead be driven by the limited size of the T helper cell pool in the context of immune homeostasis (Jameson, Reference Jameson2002). Although the quantitative details of the mutual inhibition between Th1 and Th2 responses remain unknown (as discussed below), the antagonism between these two types of T helper responses is well-established, suggesting that the host may need to allocate a finite number of T cells amongst competing demands. In particular, during co-infection the host may have to down-regulate its response toward one parasite type (e.g. a microparasite) in order to mount a potent immune response toward another, co-infecting parasite (e.g. a macroparasite) (Cox, Reference Cox2001; Page et al. Reference Page, Scott and Manabe2006). This trade-off implies that co-infected hosts face a dilemma in terms of how best to respond to co-infection; mounting too strong a response toward one parasite type may leave the host vulnerable to infection by another. Since the majority of individual hosts in many wildlife and human populations are co-infected by a wide variety of micro- and macroparasites at any one time (Hotez et al. Reference Hotez, Molyneux, Fenwick, Ottesen, Ehrlich Sachs and Sachs2006; Petney and Andrews, Reference Petney and Andrews1998), the factors affecting, and consequences of these immune allocation decisions are crucial determinants of parasite epidemiology as well as host morbidity and mortality.
Despite the abundance of laboratory studies investigating host responses toward specific co-infecting parasite combinations, to date there has been very little theoretical work aimed at synthesizing the available data into a coherent framework to predict the optimal response to co-infection. Such a framework would broaden our understanding of how different selection pressures shape the host's immune response, thereby enabling us to formulate specific hypotheses regarding how different host-parasite combinations should affect host immune allocation decision-making. An optimality framework for co-infection would also extend and complement immunologically-mechanistic theoretical analyses of phenotypic polarisation of T cell populations (e.g. Fishman and Perelson, Reference Fishman and Perelson1999; Yates et al. Reference Yates, Bergmann, Van Hemmen, Stark and Callard2000; Yates, Callard and Stark, Reference Yates, Callard and Stark2004), including work suggesting that immune responses may be fine-tuned to the dose and type of parasite, such that hosts attain global optima that encompass the full costs and benefits of mounting a given immune response (Shudo and Iwasa, Reference Shudo and Iwasa2001).
The only previous model of T helper responses to microparasite-macroparasite co-infection was based upon within-host optimization of the Th1/Th2 balance, given the severity of each infection (Graham, Reference Graham2001). The model predicted that the T helper bias of the response to co-infection would be determined by whichever infection was most detrimental to host fitness – a ‘virulence-weighted average’ that could, in principle, be tested against empirical data (Graham, Reference Graham2001). However, that model did not consider the importance of the absolute magnitude in determining the efficacy of a given immune response (i.e. its impact upon host fitness); regulatory T cells, for example, help to determine whether responses are of sufficient magnitude to clear parasites (Mills, Reference Mills2004). More importantly, by focusing purely on immune allocation decisions within a single host in isolation, this previous model was ‘static’, allowing for no feedback between the host's immune response and the abundance or infection pressure of the parasites. This is problematic because, as the efficacy of a host's response towards an individual parasite species changes, this may alter the abundance and infection pressure of that parasite among the remaining population of susceptible hosts. For example, if the magnitude of the Th1 response towards a microparasite is increased, so the host's duration of infectiousness may be expected to decrease, reducing the subsequent force of infection on the other hosts in the population and possibly altering their immune allocation decisions. Therefore, any attempt to determine the optimal immune response of a host to its parasite community has to be embedded within a population dynamic (epidemiological) framework, enabling a full appreciation of how feedback loops within the population of hosts ultimately affect the optimal immune response at the individual level (Medley, Reference Medley2002). Here, we provide a first step towards developing such a framework for co-infection. Specifically, we utilise a recently developed host-microparasite-macroparasite population dynamic model (Fenton, Reference Fenton2008) and determine how the shape of the Th1-Th2 trade-off, as well as key life-history traits of each member of this community, influence the optimal immune response of the host.
MODELLING THE OPTIMAL ALLOCATION OF THE IMMUNE RESPONSE UNDER CO-INFECTION
Basic model structure and the host's immune response
Our model is based on that of Fenton (Reference Fenton2008), in which the standard, generic host-microparasite and host-macroparasite epidemiological models of Anderson and May (Anderson and May, Reference Anderson and May1978, Reference Anderson and May1981; May and Anderson, Reference May and Anderson1978) are combined into a single host-microparasite-macroparasite model. The structure of this model is described in detail in the Appendix, and all parameters are defined in Table 1.
State variable and parameter definitions

Although host immune responses are not explicitly modelled, the model does incorporate key parameters that may be used as proxies for the magnitude of the immune response toward each parasite type. For example, the magnitude of the Th1 immune response towards the microparasite is captured by the recovery rate parameter (σ); large values of σ reflect high clearance rates, indicative of a strong Th1 immune response. For convenience we assume that, once developed, immunity to the specific microparasite strain being considered is lifelong, so we adopt an ‘SIR’ (Susceptible-Infected-Recovered) framework rather than ‘SIS’ (Susceptible-Infected-Susceptible); it is possible that alternative formulations may result in different predictions from those presented here. The magnitude of the Th2 response towards the macroparasite may be captured by two parameters: the adult parasite mortality rate (μ) and the inverse of the adult parasite fecundity rate (1/λ); large values of either of these parameters reflect a strong Th2 immune response. In general, the results of assuming the host's Th2 response affects macroparasite fecundity (λ) do not qualitatively differ from those where the Th2 response affects macroparasite survival (μ). Furthermore, restricting the model to allow hosts to dynamically alter μ during the period of co-infection (i.e. during the ‘I’ stage) merely reduces the relative investment in the Th2 response, without altering the qualitative predictions of the model. Therefore, for simplicity, we just present results of the analyses assuming the host's Th2 response affects macroparasite survival and is fixed throughout the duration of the host's lifespan. Finally, we restrict our analyses to regions of parameter space where both parasite types (both the micro- and macroparasite) are endemic within the host population for all values along the μ-σ trade-off curve (or, indeed, for maximal values of μ and σ under single infection) and neither parasite can be eradicated by the collective action of the host population (i.e. the basic reproduction ratio, R 0, for both parasites is always greater than 1 even under maximal immune responses), thereby ensuring that we are truly examining the evolution of host immune responses under co-infection.
Defining trade-offs within the host's immune response in the model
Our model framework allows us to consider how a trade-off between the Th1 and Th2 arms of the immune response would affect the epidemiology, prevalence and/or abundance of the component parasite species. Firstly, we consider the situation in which each parasite infects in isolation (i.e. there is no co-infection). Under these conditions the host is assumed to mount a maximal immune response towards each species (Fig. 1). Therefore, under single infection the host can impose a maximal mortality rate on the macroparasite (μMAX) and a maximal clearance rate on the microparasite (σMAX). These correspond to maximal Th2 and Th1 responses, respectively. Furthermore, in the absence of a trade-off within the host's immune system, we would expect co-infected hosts to mount full Th1 and full Th2 responses simultaneously and so the optimal response, {μ*, σ*}, under co-infection is simply the combination of both maximal single responses {μMAX, σMAX} (denoted by ‘*’ in Fig. 1).
Conceptual diagram of potential trade-offs between investment in the Th1 (anti-microparasite) and Th2 (anti-macroparasite) arms of the host immune response, represented by the microparasite clearance rate (σ) and the macroparasite mortality rate (μ) respectively. Under single infection, the host is assumed to invest maximally in the appropriate immune response (e.g. under infection by the microparasite alone, optimal investment in the Th1 response, σ*=σMAX; under infection by the macroparasite alone, optimal investment in the Th2 response, μ*=μMAX). Hence, in the absence of a trade-off, the host would be expected to invest optimally in both Th1 and Th2 responses under co-infection (denoted by the ‘*’). However, given a trade-off (represented by the dotted lines), the optimal response, {μ*, σ*}, will lie somewhere along the trade-off curve, the exact position determined by host, microparasite and macroparasite life-history traits.

As described above, there is a trade-off between the ability of the host to mount a Th1 response and its ability simultaneously to mount a Th2 response. At this stage, we assume that the efficacy of the immune response mounted against a parasite under co-infection is always less than or equal to the efficacy of response against the parasite under single infection. It is possible, however, for co-infection to result in an increased host response. For example, some parasite species manipulate the immune response to promote survival (e.g. via induction of regulatory T cells; Mills, Reference Mills2004), whereas under co-infection such manipulation may be disrupted, allowing the host to mount a more effective response against the parasite. However, for this paper we concentrate on the scenario of an antagonistic interaction between the Th1 and Th2 arms of the immune response that can render the response to co-infection less effective than responses to single species infection.
To our knowledge, the functional form of a Th1/Th2 trade-off during co-infection has not yet been determined in vivo for any empirical system. Several obstacles have slowed description of these functions to date. For example, because their interests lie elsewhere, researchers conducting immunological studies of co-infection tend not to undertake quantitative exploration of Th1/Th2 covariance and virtually never consider covariance of microparasite clearance rates with macroparasite mortality rates. Such analyses are feasible in principle, perhaps via collaboration between empiricists and mathematicians/statisticians, and we would encourage work in this direction.
Discovery of phenotypic trade-off curves is non-trivial even in laboratory systems, as illustrated with data from malaria-filaria co-infection in Fig. 2. In this empirical example, laboratory mice with chronic filarial (Litomosoides sigmodontis) infection were given an acute malaria (Plasmodium chabaudi chabaudi) co-infection. Co-infected mice either experienced exacerbated malarial disease or else allowed microfilariae to circulate, depending upon the strength of the systemic cytokine response mounted, as described previously (Graham et al. Reference Graham, Lamb, Read and Allen2005). The antibody data from those experiments (which are previously unpublished) allow exploration of the Th1-Th2 antagonism in co-infected mice, as follows. After twenty days of co-infection, total serum IgG1 and IgG2a antibodies were measured using ELISA. These antibody isotypes may be used as markers of Th1/Th2 bias in mice because the switch to the IgG2a isotype is directly promoted by the signature Th1 cytokine interferon (IFN)-γ, while IgG1 is promoted by Th2-driving interleukin(IL)-4 (Snapper et al. Reference Snapper, Finkleman and Paul1988a, Reference Snapper, Peschel and Paulb). Note that although helminths do induce regulatory cytokines such as IL-10 (Maizels et al. Reference Maizels, Balic, Gomez-Escobar, Nair, Taylor and Allen2004) in addition to IL-4, IgG1 isotype switching is not under the influence of IL-10 in mice (Shparago et al. Reference Shparago, Zelazowski, Jin, McIntyre, Stuber, Pechana, Kehry, Mond, Max and Snapper1996).
Empirical data illustrating the difficulty and yet future promise of demonstrating Th1/Th2 trade-offs. The data come from experiments described in (Graham et al. Reference Graham, Lamb, Read and Allen2005). Each point represents a malaria-filaria co-infected mouse. A) A positive correlation between Th1-associated and Th2-associated antibodies (IgG2a and IgG1, respectively), indicating that individual variation in immune response strength may obscure phenotypic trade-offs; B) Residuals of Th1 antibodies once overall strength of immune response was controlled for statistically, to show remaining variation in Th1/Th2 immune bias; and C) Residuals of Th1 antibodies as predictor of microparasite clearance rate, demonstrating the functional relevance of residual Th1/2 bias.

When the Th1-associated IgG2a and Th2-associated IgG1 data for co-infected mice were plotted together (Fig. 2A), they showed no evidence of a trade-off. Instead, a significant positive correlation was evident, suggesting that variation among mice in total immune responsiveness was predominant – i.e. an effect of individual ‘quality’ and/or differential induction of immunomodulatory cytokines such as IL-10 or transforming growth factor (TGF)-β (Maizels et al. Reference Maizels, Balic, Gomez-Escobar, Nair, Taylor and Allen2004). Statistically controlling for this effect revealed substantial residual variation in Th1/Th2 allocation among co-infected mice (Fig. 2B). The functional relevance of this variation in allocation to Th1 versus Th2 arms of the immune response is shown in Fig. 2C, in which the residual Th1 antibody is plotted against malaria clearance rate (days of patency−1): the more Th1-biased a co-infected individual's response, the more quickly it cleared its malaria parasites (regression slope=0·040±0·018; P=0·015). (Data on clearance of filarial worms in these mice were insufficient to generate an empirical equivalent of Fig. 1.)
Thus, these data indicate that different Th1/Th2 allocation decisions made by co-infected individuals have functional consequences, and indeed that laboratory mice, despite extensive inbreeding, are sufficiently variable to give data across a range of parameter space. In addition, the data suggest that variation in overall immune responsiveness may need to be taken into account in order to reveal phenotypic trade-offs between the ability of a host to clear microparasites versus macroparasites. For all of these reasons, we are hopeful that further experimental and statistical work will reveal the shapes of trade-offs between μ and σ – or Th2 and Th1 – in many co-infection systems. We revisit empirical issues in the Discussion (below).
Due to the lack of current empirical information on the functional form of the Th1/Th2 trade-off, we deliberately keep our analyses highly generic, rather than tailored to any specific host-microparasite-macroparasite system, and explore the qualitative consequences of a range of possible trade-off curve shapes (shown by the dotted lines in Fig. 1) for the optimal immune allocation decision of the host. In the simplest scenario, there may be a finite population of precursor T cells that may differentiate into either Th1 or Th2 cells as needed. In this scenario, we would expect a linear trade-off curve, such that cells which differentiate into Th1 cells are not available to become Th2 cells, and vice versa. Conversely, the trade-off curve may be concave (Fig. 1). This scenario may occur if T cells are only limiting over a relatively small spatial scale within the host (or if the cytokines that polarise T helper populations only work on the local scale). In this case, providing the two parasites occupy separate spatial locations within the host, the Th1/Th2 trade-off will be less pronounced. In the extreme case where the two parasites occupy completely isolated locations within the host, there will be no localised T cell limitation (and/or no scope for cytokine-mediated antagonisms) and the optimal immune response will once again be the combination of maximal responses: {μ*, σ*}={μMAX, σMAX}. Finally, the trade-off curve may be convex (Fig. 1). This scenario may occur if there is strong interference between the two arms of the immune response generating a positive feedback, so that as the host mounts an immune response in one direction (e.g. towards a Th2 response), the expansion of associated cytokines stimulates further growth towards that response, biasing the immune system away from the opposite direction (as explored by Fishman and Perelson (Reference Fishman and Perelson1999) and Yates et al. (Reference Yates, Bergmann, Van Hemmen, Stark and Callard2000, Reference Yates, Callard and Stark2004), for example).
Defining the optimal immune response under co-infection
Here we adopt a simple, optimality approach to provide an initial insight into the factors affecting the allocation of host resources towards the Th1 and Th2 arms of immunity during co-infection when epidemiological feedbacks are operating. To do this we define the fitness of the host in terms of its mean lifetime reproductive success, Φ (see Table 1 for variable and parameter definitions; see Appendix for further details):

where Ω=b+βVI*+αWM S* (the average net rate of loss of hosts susceptible to the microparasite), M S*, M I* and M R* are the equilibrium values of the mean macroparasite burdens in Susceptible, Infected, and Recovered hosts, respectively, and I* is the equilibrium abundance of microparasite-infected hosts, calculated for a given set of parameter values under the specified trade-off between μ and σ. That is, for a given rate of macroparasite mortality μ, the corresponding rate of microparasite clearance, σ, can be calculated from the assumed trade-off relationship. This pair of values is then used to calculate the equilibrium values mentioned above and, hence, the mean lifetime reproductive success, Φ. Therefore, the average fitness of an individual depends on the combination of all host, microparasite and macroparasite parameters (e.g. parasite virulence and transmission rates and host reproduction and mortality rates). Crucially, Φ varies in response to changes in adult macroparasite mortality rate (μ), and the corresponding value of σ as determined from the assumed trade-off (Fig. 3). Therefore Fig. 3 shows how the allocation of resources to the different arms of the immune response determines the average fitness of individuals in the host population. We then define the optimal strategy {μ*, σ*} as the combination of μ and σ that maximises Φ (denoted by the dotted lines in Fig. 3).
Fitness landscapes showing how mean lifetime reproductive success, Φ, varies with investment in the Th2 response (as measured by macroparasite mortality rate, μ). The optimal investment in the Th2 response, μ*, is given as the value of μ that gives the highest value of Φ; the corresponding investment in the Th1 response, σ*, is given from a linear trade-off curve between μ and σ (e.g. Fig. 1). Parameter values are: βV=0·005, a=0·1, b=0·01, k=1, γ=0·3, λ=100, αW=0·001, αV=0·1. A) a sharply peaked fitness curve, indicative of strong selection pressure, produced when βW=1×10⁻⁷ and B) a flat fitness landscape, indicative of very weak selection pressure, produced when βW=8×10⁻⁶.

It should be noted that the shape of this fitness curve also defines the strength of selection; if the fitness curve is sharply peaked (e.g. Fig. 3A) then departures from the optimal strategy selection are very costly, and there is strong selection for the optimal response. If the fitness curve is very flat around the optimum (e.g. Fig. 3B) then departures from the optimum are not costly and selection is very weak (i.e. although there is a single optimum strategy it may take a very long time to achieve). This model therefore improves upon the arbitrary fitness function that was used in the previous model of optimal immune responses to co-infection (Graham, Reference Graham2001); in the present model the shape of the fitness surface naturally emerges from the epidemiological relationships between the host, microparasite and macroparasite. In what follows we concentrate primarily on just the optimal strategy, regardless of the strength of selection, but will consider the implications of such evolutionary dynamics in the future. Furthermore, the model adopts a simple optimality approach, in which all individuals in the population are assumed to play the same strategy (i.e. they all have the same values of μ and σ), ignoring any potential conflict between the population optimum and that of each individual. In the Discussion we consider the implications of this assumption, and describe alternative approaches that could be adopted in future to address the issue of between-individual variation in immune responses. Finally, we emphasise that at this stage we are purely interested in broad predictions of the model and so present results for arbitrary parameter values that are not based on any host, microparasite or macroparasite species in particular; we will parameterise and test our predictions in the future using the rodent-malaria-nematode lab system described above and in Graham et al. (Reference Graham, Lamb, Read and Allen2005).
RESULTS
Impact of trade-off shape on the optimal immune response
Fig. 4 shows how altering the functional form of the Th1/Th2 trade-off affects the predicted optimal immune response, for increasing microparasite transmission rates (βV). Firstly, it can be seen that, regardless of the trade-off shape, as microparasite transmission rate increases so the optimal allocation towards the Th2 arm of the immune response (as measured by the adult macroparasite mortality rate, μ) decreases, with a corresponding increase in allocation towards the Th1 arm (measured by the microparasite clearance rate, σ). Intuitively this makes sense, since as βV increases so hosts face an increasing risk of microparasite infection. Therefore, on average, hosts should invest more strongly in an effective Th1 response to be better able to clear a microparasite infection, sacrificing the strength of their Th2 responses. Hence, the immune response should be increasingly Th1-biased in the face of microparasites with high transmission rates.
Impact of trade-off shape between σ and μ on the optimal investment in the Th1 and Th2 arms of the immune response under different values of microparasite transmission rate, βV. Optimal investment values are expressed relative to the maximal value assumed under single infection (e.g. μ*/μMAX and σ*/σMAX); values approaching 1 indicate very high levels of investment in that arm of the immune response, with correspondingly low values of investment in the alternative response. Parameter values are: βW=5×10⁻⁶, βV=0·005, a=0·1, b=0·01, k=1, γ=0·3, λ=100, αW=0·001, αV=0·1.

A second result is that as the trade-off between Th1 and Th2 responses moves from being convex (Fig. 4A) to linear (Fig. 4B) to concave (Fig. 4C), so the optimal allocation to both arms of the immune response increases (i.e. the optimal immune response moves towards the upper right hand region of Fig. 1). Under a convex trade-off we would predict polarisation of the immune response, such that the host should invest relatively highly in one arm of the response under co-infection, at the expense of the other (Fig. 4A). Increasing concavity of the trade-off allows the host to allocate substantial resources to both arms of the immune response simultaneously, without sacrificing either component in favour of the other (see Fig. 1). As suggested earlier, under extreme concavity, there is effectively no trade-off, and the optimal strategy is once again the combination of maximal responses: {μ*, σ*}={μMAX, σMAX} (Fig. 1). In what follows, we focus simply on linear trade-offs to illustrate how different parameters affect the optimal immune response, but bear in mind that the quantitative values predicted would be lower if there was a convex trade-off and higher if there was a concave trade-off.
Impact of host, microparasite and macroparasite life-history parameters on the optimal immune response
Using our model framework we can assess how different host, microparasite and macroparasite life-history traits influence the optimal Th1/Th2 response of the host. At present we simply concentrate on the impact of each trait in isolation; analysis of potential interactions between traits would be of considerable interest, but are outside the scope of the present paper.
In the following figure we present the results for the optimal investment in the Th2 response, as measured by the macroparasite mortality rate (μ*); the corresponding values for σ* are inversely related to these due to the assumed linear trade-off (i.e. high μ* implies low σ* and vice versa). We express this optimal investment in the Th2 response relative to the maximum possible value attainable in the absence of a trade-off (or under single infection; μMAX), so values approaching 1 show very high degrees of Th2-biased immunity, with correspondingly low values of Th1 investment.
The model shows that the optimal immune response is greatly affected by many host, micro- and macroparasite life-history traits (Fig. 5). As described above, increasing the microparasite transmission rate (βV) results in a decrease in investment in the Th2 response in favour of an increased Th1 response. Conversely, increasing either macroparasite transmission rate (βW) or fecundity (λ) both tend to result in increased investment in the Th2 response, to better combat the increased pressure of macroparasite transmission. Similarly, increasing the mortality rate of the macroparasite's free-living stages (γ) results in a decreased infection pressure from macroparasites, and so selects for decreased investment in the Th2 immune response.
Impact of host, microparasite and macroparasite life-history traits on the optimal investment in the Th2 (anti-macroparasite) arm of the immune response, under an assumed linear trade-off with the Th1 (anti-microparasite) arm of the immune response. As in Fig. 4, optimal investment values are expressed relative to the maximal value assumed under single infection (e.g., μ*/μMAX). Unless otherwise stated, parameter values are: βW=5×10⁻⁶, βV=0·005, a=0·1, b=0·01, k=1, γ=0·3, λ=100, αW=0·001, αV=0·1.

While the above results are intuitive, the model predicts that increasing macroparasite per capita virulence (the additional host mortality due to infection by each individual macroparasite; αW) appears to select for decreased investment in Th2 immunity, whereas increasing microparasite transmission (αV) appears to select for increased investment in the Th2 immune response (and, therefore, a corresponding decrease in investment in Th1 immunity). These apparently counter-intuitive results arise because our measure of fitness (mean lifetime reproductive success) considers the average investment in Th1 and Th2 immune responses across the whole host population. Since increasing microparasite (or macroparasite) virulence results in death not only of the host, but also of the infecting parasite, the more virulent the parasite the lower the force of infection on the remaining population. Similar results are observed from a population dynamics perspective, where the greatest degrees of host population suppression are predicted to be achieved by parasites with relatively low per capita virulences; too highly virulent parasites die out before they have a chance to transmit (Anderson, Reference Anderson1980; McCallum and Dobson, Reference McCallum and Dobson1995). Therefore, due to the epidemiological feedback on the size of the parasite population, an average individual would be unlikely to experience infection by a highly virulent parasite and so the optimal strategy is for the immune system to be naturally biased towards the other, more prevalent parasite. This result illustrates the importance of placing within-host optimization problems into an epidemiological context (Medley, Reference Medley2002). Although our present model takes into account the epidemiological feedback between the host's immune response and the parasites' forces of infection, at the level of the individual host it would be expected that virulent parasites should receive immunological priority during co-infection (Graham, Reference Graham2001). As described in detail in the Discussion, a more complete theoretical framework is ultimately needed that will bring together both the optimal strategy at the individual level and the population-level consequences of those responses.
A related pattern to that described above is seen when k of the negative binomial distribution of the macroparasite population is increased, resulting in increased investment in the Th2 response. This parameter determines the degree of aggregation of macroparasites across the host population. At low values of k, parasites are highly aggregated, resulting in very few hosts harbouring the majority of infections. Therefore, death of these heavily infected hosts leads to a large reduction in size of the macroparasite population, and therefore a low average investment in Th2 responses across the host population. However, as k increases, so more hosts on average become infected and so Th2 investment becomes more pronounced.
Finally, the model is able to predict how optimal immune allocation will vary in response to biological parameters for which we may not be able to make a priori predictions. For example, increasing host reproductive rate (a) leads to a decrease in Th2 investment until, at sufficiently high values of a, Th2 investment should be negligible, and Th1 investment maximal. Increasing host reproduction increases the transmission potential of both parasite types, but microparasite transmission increases linearly with increasing host density, whereas macroparasite transmission increases sub-linearly (May and Anderson, Reference May and Anderson1979). Therefore microparasite infection becomes a bigger threat to hosts than macroparasite infection and so Th1 investment increases as host reproduction increases. Finally, increasing the host's background mortality rate (b) has little initial impact on the optimal allocation of resources. At sufficiently high values of b, investment in the Th1 response becomes increasingly favoured over investment in the Th2 response. This is because at high b values hosts are, on average, very short lived and so do not have time to accumulate high macroparasite burdens. Therefore microparasite infection becomes a much more significant factor to host fitness and higher levels of investment in the Th1 response are selected for.
DISCUSSION
Here we have presented an optimality model that provides a first step towards understanding the optimal allocation of host resources towards either an anti-microparasite Th1 immune response or an anti-macroparasite Th2 immune response in the face of co-infection, within an epidemiological framework. The work presented here sets a challenging research agenda for both empiricists and theoreticians interested in simultaneous immune responses to micro- and macroparasitic infections. We begin by outlining the sorts of empirical studies that would help define the functional form of the Th1-Th2 trade-off. Later, we discuss the model results in more detail, and also highlight future approaches to the mathematical modelling that would allow the scale of inference about optimality to move from the level of the host population to that of the host individual.
Despite considerable published research on immunology and parasitology under single or co-infection, empirical data on the functional form of any Th1/Th2 trade-off are lacking, as described in the model development section above. For example, cytokines associated with Th1 versus Th2 (Abbas et al. Reference Abbas, Murphy and Sher1996) and regulatory immune responses (Mills, Reference Mills2004; Maizels et al. Reference Maizels, Balic, Gomez-Escobar, Nair, Taylor and Allen2004) are now routinely measured in immuno-parasitological studies, and the effect of co-infection upon parasite clearance is often observed as well (Cox, Reference Cox2001; Page et al. Reference Page, Scott and Manabe2006). The next step of quantitatively relating one parameter to another is rarely taken. Specifically, we suggest that it is crucial to quantify the functional consequences of immune responses (e.g. microparasite clearance, macroparasite mortality or reduced macroparasite fecundity) in relation to the abundance of antibodies, T cells and/or cytokines, as we have attempted to illustrate with the malaria clearance data in Fig. 2C. A complementary statistical analysis of how helminth mortality rate depends upon the serum concentration of a Th2 effector such as IgE (Snapper et al. Reference Snapper, Finkleman and Paul1988a) would address the functional relevance of variation in Th2 bias during co-infection. Ideally, researchers would analyse covariance between the rate of clearance of microparasites and the mortality rate of macroparasites in co-infected hosts, to obtain empirically-grounded equivalents of the concepts diagrammed in Fig. 1. Such data would most directly map onto the various parameters used in standard parasite epidemiology models (Anderson and May, Reference Anderson and May1978,Reference Anderson and May1981), which are likely to form the basis of future models of parasite co-infection (Fenton, Reference Fenton2008).
If, however, data on parasite killing are incomplete (as was the case in the malaria-filaria co-infection work (Graham et al. Reference Graham, Lamb, Read and Allen2005) in which macroparasite data were not obtainable), then covariance between immunological measures of Th1 versus Th2 responses might be informative. In particular, if the relationship between these immunological measures and their functional consequences (i.e. degree of worm killing, or microparasite clearance) are known from single-species infections (e.g. Graham, Reference Graham2001) then it may be possible to estimate the functional consequences of a Th1/Th2 trade-off from observed reductions in these immunological measures under co-infection. As discussed previously, the difficulty remains that individual hosts may vary in the overall investment in their immune response, such that phenotypic data on Th1 and Th2 immune responses are positively correlated (Fig. 2A) and so statistical correction for individual host variation in overall response magnitude would be required (e.g. Fig. 2B).
Future empirical work will also need to take into account a variety of factors such as anatomical location of both parasite species (Lamb et al. Reference Lamb, Graham, Le Geoff and Allen2005) as well as infection chronicity and dose (Bleay et al. Reference Bleay, Wilkes, Paterson and Viney2007). Indeed, there will be system-specificity to many conclusions of empirical studies – it is extremely unlikely that a uniform trade-off function will apply to all co-infection systems. Nevertheless, we believe it is possible to collect such data using current laboratory systems, and our model provides an excellent framework within which to interpret those data and predict expected patterns of immune allocation for those specific systems. For example, our model showed that the optimal allocation decision depends quantitatively on the functional form of the underlying trade-off between these two arms of the immune response (Fig. 4). Under increasingly concave trade-offs it is possible to invest relatively strongly in both types of immune responses, without compromising either. Such concave trade-offs may be expected when limitations on T cell abundance are relatively localised within the host or if resources are not limiting. Therefore, we would predict that if the microparasite and macroparasite occupy physically distinct locations within the host, then the host would be expected to mount relatively strong immune responses towards both co-infecting parasites. However, if the parasites occupy similar physical locations, or if there is interference between the two arms of the immune response, such that initial investment in one response stimulates further investment into that response, then we would predict that overall the host would invest comparatively less in both arms of the immune response. Furthermore, when there is interference between the two arms of the immune response (i.e. a convex trade-off), we would also predict that there should be polarisation of the immune response, such that the host should invest relatively heavily in one arm of the immune response at the expense of the other. Such predictions can in principle be tested against empirical data from a diverse range of co-infections; ultimately, empirical and theoretical studies might tackle the operation of Th1-Th2 trade-offs during co-infection in the field, although such an ambitious goal is arguably best left until the operation of trade-offs in model systems in the laboratory is much better understood.
A primary result of the mathematical analysis is that the different shapes of the trade-off curve (Fig. 1) did not qualitatively change the effect of increasing microparasite transmission rate on relative resistance to each parasite (Fig. 4). The quantitative differences in slope could have important practical consequences at the individual as well as whole-population level. For example, for a given rate of microparasite transmission (say βV=0·004 in Fig. 4), the relative resistance of co-infected hosts to macroparasites (top panels) can vary from a 10% reduction (in the case of the concave trade-off in panel C) to a 60% reduction (in the case of the convex trade-off in panel A) in response efficacy, compared to hosts infected with macroparasites alone. This should, in turn, affect the prevalence of co-infection, and it would be of interest to discover which trade-off scenario is most consistent with the prevalence observed in a given population. Indeed, it will be important in future work to relate empirical findings on Th1/Th2 trade-offs to empirical data on geographical variation in forces of infection by both micro- and macroparasites (e.g. Booth et al. Reference Booth, Vennervald, Kenty, Butterworth, Kariuki, Kadzo, Ireri, Amanga, Kimani, Mwatha, Otedo, Ouma, Muchiri and Dunne2004).
Our model is primarily epidemiologically-based, rather than immunologically, and so makes a number of simplifying assumptions concerning the nature of the immune response to each parasite type. Firstly, the model assumes that once recovered from microparasitic infection the host has life-long immunity to that microparasite strain (i.e. the model adopts an SIR framework). Other scenarios are possible though, including a gradual waning of immunity over time (an SIRS framework) or immediate loss of immunity to that strain (an SIS framework). Using an adaptive dynamics framework (see below), Miller, White and Boots (Reference Miller, White and Boots2007) showed that the evolutionary investment in immunity against a microparasite under single infection can vary qualitatively and quantitatively depending on the rate of loss of immunity. How these predictions are altered in the presence of a co-infecting macroparasite remains to be seen. Secondly, our model assumed that hosts did not dynamically alter their Th1/Th2 allocation in response to their infection status; the macroparasite mortality rate (μ) was fixed regardless of the infection class of the host (i.e. whether it was susceptible to, infected by or recovered from the microparasite). Allowing hosts to dynamically alter investment in the Th2 response during the period of co-infection (i.e. such that μI – the macroparasite clearance rate during the period of infection with the microparasite – could differ from μS and μR) simply reduced the optimal investment in the Th2 response (with a corresponding increase in the Th1 response) during the period of co-infection, without altering the qualitative predictions of the model. This is because during the ‘S’ and ‘R’ stages the model effectively reduces to a single infection macroparasite framework, and the hosts can invest maximally in their Th2 response. However, during the ‘I’ stage the host is co-infected and it pays to invest highly in the Th1 response, clear the microparasite infection as soon as possible, and revert to the single infection R stage where it can once again invest maximally in the Th2 response. Hence, the model suggests that if hosts are able to perfectly adjust their immune allocations in response to changes in their infection status, then hosts should down-regulate their Th2 allocation during bouts of co-infection and the up-regulate them again once the microparasite has been cleared.
By incorporating the full epidemiological feedback between hosts, microparasites and macroparasites, our model was also able to show how their respective life-history traits influence the immune allocation decisions. Many of the predictions of the model were intuitive, such that as infection pressure by one parasite (i.e. transmission rate) increases, so investment towards the relevant arm of the immune response should increase (e.g. increased microparasite transmission rate, βV, selects for increased investment in Th1 immunity). Furthermore, the model also predicted how the optimal immune allocation decision would vary in response to changes in other parameters for which we would not necessarily be able to make a priori predictions. In particular, the model showed that as either host reproductive rate (a) or host background mortality rate (b) increases so the immune response should become increasingly Th1 biased. These patterns arise due to the way in which parasite exposure and accumulation vary with host density and life-span for the two parasite types, tending to lead to high microparasite exposure relative to macroparasite exposure at high densities or within short-lived hosts. These predictions may be tested through comparative studies from field data where, all else being equal, we would predict relatively higher investment in Th1 responses in fast reproducing, short-lived host species compared to long-lived species with low reproductive rates. Similarly, within a host species, we may predict relatively higher investment in Th1 responses for host populations living in stressful environments where there is a high extrinsic mortality rate (e.g. populations with high predation pressure) than for populations in benign environments where mean life-span is longer.
Finally, our model predicted apparently counter-intuitive responses to parasite virulence: as virulence of one of the parasites increased, so investment in the corresponding immune response should decrease (e.g. increasing microparasite virulence, αV, resulted in decreased investment in the Th1 response). This was due to the epidemiological feedback within the model framework; death of an infected host results in a reduction in infection pressure on the remaining hosts in the population, and so the lower the average investment in immune response towards that parasite across the whole population. It would still be expected that an individual host, upon infection by a highly virulent parasite, should increase investment in the appropriate immune response. This conflict between individual and population optima forms the core of the future theoretical research agenda that arises from this work, as follows.
The optimality approach adopted here takes a restrictive view of evolution, which implies that all individuals in the population play the same strategy (i.e. they all have the same values of μ and σ). Clearly, however, there may be a conflict between the population optimum and that of each individual; hence, a more complete analysis that allows for this conflict is ultimately needed. One possible approach to tackle this issue would be to construct an individual based model and track the distribution of evolutionary responses of all individuals in the population. An alternative would be to adopt a game-theory approach, in which the optimal (strictly, evolutionarily stable) strategy is defined as one that is unbeatable by any other strategy. Similar approaches, using an adaptive dynamics framework, have previously been adopted to address the much simpler issue of the evolutionarily stable investment in immunity towards microparasites alone (Bowers, Reference Bowers1999; Boots and Bowers, Reference Boots and Bowers1999, Reference Boots and Bowers2004; Miller et al. Reference Miller, White and Boots2007). These models take into account the competitive nature of evolution by considering whether a novel host ‘strain’ arising by mutation can invade and replace existing host strains; if so, then evolution will proceed in the direction of the new strain's life-history traits. Both of these approaches would be considerably more complex for the issue of parasitic co-infection and are beyond the scope of the present paper. Therefore, the present optimality approach, although limited, provides an important first step. It is hoped that by building on this framework and conducting the experiments outlined above to quantify the functional shape of any Th1/Th2 trade-off, we can truly make progress in understanding how various host, microparasite and macroparasite life-history traits combine to determine the evolution of host responses to co-infection.
ACKNOWLEDGEMENTS
The authors thank the BBSRC and Wellcome Trust for funding the empirical work, and the BBSRC for fellowship support of ALG.
APPENDIX A: THE MICROPARASITE-MACROPARASITE CO-INFECTION MODEL
Our co-infection model is based on the Susceptible-Infected-Recovered (SIR) microparasite model of Anderson and May (Reference Anderson and May1981):


and the macroparasite model of Anderson and May (Reference Anderson and May1978):


where parameters are as defined in Table 1. Note that we use subscripts ‘V’ (for ‘virus’ although we stress that this refers to a generic microparasite, rather than specifically relating to viruses) and ‘W’ (for ‘worm’) to distinguish between parameters that may apply to either the microparasite or macroparasite respectively.
Combining these models, and keeping track of the mean macroparasite burdens in hosts susceptible to, infected by and recovered from the microparasite (M S, M I and M R respectively) produces the hybrid host-microparasite-macroparasite model given in Fenton (Reference Fenton2008):


where N=S+I+R and Γ=μ+αW.
Given this framework we define host fitness as the average lifetime reproductive success of an individual in the host population, Φ, which we define as follows. A host individual is uninfected by the microparasite, on average, for T S time units, during which it reproduces at rate ρS per time unit. A host is infected by the microparasite on average for T I time units, during which it reproduces at rate ρI per time unit. Finally, a host is recovered from microparasite infection for T R time units, during which it reproduces at rate ρR per time unit. Therefore the per capita rate of increase of an average host individual throughout its lifetime (i.e., the average lifetime reproductive success of an individual in the host population, Φ) is:

Following previous models (Boots and Bowers, Reference Boots and Bowers2004; Miller et al. Reference Miller, White and Boots2007) these values can be derived directly from the model equations above to give:

where Ω=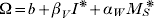 . Inserting these values into equation A1 gives the value of Φ presented in the main paper.



