The New Zealand (NZ) dairy industry is predominantly based on a grazed, pasture-based out-door farming system with cows typically being milked through the months of August to May inclusive, but with some variation in this reflecting latitude and seasonal pasture growth. The industry is dominated by Holstein-Friesian and Jersey cattle, with Holstein-Friesian × Jersey (HF × J) cross cows now gaining in favour.
The ability of a dairy cow to resist contagious disease is in part related to the activity of its immune system. This system consists of a variety of mechanisms and processes, and these are capable of both non-specifically and specifically targeting invading microorganisms (Ingvartsen & Moyes, Reference Ingvartsen and Moyes2013). Pattern recognition receptors (PRRs) are known to play an important role in the innate, or non-adaptive immune response (Janeway & Medzhitov, Reference Janeway and Medzhitov2002), as they detect the presence of pathogens that breach an animal's surface defences, but there is also growing evidence to suggest that PRRs play a role in adaptive, or specific immune responses (Werling & Jungi, Reference Werling and Jungi2003).
The toll-like receptors (TLRs) are a family of mammalian PRRs and recognise highly conserved structural motifs known as pathogen-associated molecular patterns (PAMPs) that are shared by pathogens, but distinguishable from the host's molecules. In the TLR family, TLR4 is known for recognising lipopolysaccharide (LPS), a component of many Gram-negative bacteria. The gene that encodes bovine TLR4 (TLR4) is polymorphic, with most of the variation located within the coding region (White et al. Reference White, Taylor, Abbey, Gill and Womack2003) where it may affect PAMP recognition. Accordingly TLR4 variation may underpin variation in susceptibility to diseases that affect the productivity of dairy cattle.
In this context, investigation of the effect of bovine TLR4 variation on immunity and cattle productivity has been focused on susceptibility to mastitis (Sharma et al. Reference Sharma, Leyva, Schenkel and Karrow2006) and paratuberculosis (Sharma et al. Reference Sharma, Abo-Ismail, Schenkel, You, Verschoor, Pant and Karrow2015). There are a number of studies reporting associations between TLR4 polymorphism and milk production in dairy cows. Sharma et al. (Reference Sharma, Leyva, Schenkel and Karrow2006) described an association between TLR4 and lactation persistency in Canadian dairy cattle, while in Irish cattle Beecher et al. (Reference Beecher, Daly, Childs, Berry, Magee, McCarthy and Giblin2010) described an association between variation in TLR4 and milk fat and protein percentage in late lactation. In Iranian Holstein cattle Noori et al. (Reference Noori, Mahdavi, Edriss, Rahmani, Talebi and Soltani-Ghombavani2013) described an association between TLR4 exon 3 variation, and somatic cell score (SCS) and milk-related traits (305-day milk yield, breeding value for milk yield and lower fat percentage), while Zhu et al. (Reference Zhu, Wang, Xing, Yang and Mao2016) have described how polymorphisms of the TLR4 gene influences milk production traits (fat content and total solids) in Chinese Holstein cows.
In this study, we used a polymerase chain reaction-single stranded conformational polymorphism (PCR-SSCP) analysis to investigate a variable region of TLR4 in 402 NZ Holstein-Friesian × Jersey (HF × J) cross cows, and whether this variation was associated with some milk traits.
Materials and methods
All research at Lincoln University involving dairy cows was carried out in accordance with the Code of Welfare for Dairy Cattle, issued by the Minister for Primary Industries (Section 75 and 76 of the Animal Welfare Act 1999 -New Zealand Government).
Cows and blood samples
The study involved 402 NZ HF × J-cross cows of three to nine years of age. These cows were exclusively grazed outdoors on perennial ryegrass-white clover pastures at the Lincoln University Dairy Farm. A sample of venous blood was collected from each cow onto FTA cards (Whatman BioScience, Middlesex, UK) and these cards stored at room temperature, in the dark, until analysed.
Milk sample collection and phenotype measurement
The cows were milked in the early morning and then again in the middle of the afternoon. Their daily milk yield (MY) in kilograms wet-weight was measured using Tru-test milk meters (Tru-test Ltd, Auckland, NZ).
Six milk samples (from both the morning and afternoon milking) were collected over September to February of 2015 (corresponding to the spring and summer seasons) and analysed for fat percentage (FP) and protein percentage (PP) using Fourier-Transform Infra-Red Spectroscopy (MilkoScan FT 120 Foss, Hillerød, Denmark). Individual cow FP and PP measurements were averaged over the recording period and these averages were used in the association analyses.
Genotyping of bovine TLR4
Bovine TLR4 was genotyped using PCR-SSCP analysis. Primers (5′-1566TCAGGTGCTGAATATGAGTCA1586-3′ and 5′-2064CCAGTCTTCATCCTGGCTC2046-3′) were designed based on a bovine TLR4 sequence (GenBank AY297040) to amplify an estimated 499-bp fragment of exon 3. This is probably the most variable region of TLR4, with 11 SNPs being reported to date (White et al. Reference White, Taylor, Abbey, Gill and Womack2003). Primers were synthesized by Integrated DNA Technologies (Coralville, IA, USA).
Genomic DNA for PCR amplification was purified from a 1·2 mm punch of the dried blood using an extraction method described by Zhou et al. (Reference Zhou, Hickford and Fang2006) and amplification was undertaken in 15-μl reactions containing the purified DNA, the primers at 0·25 µm, 150 µm dNTPs (Bioline, London, UK), a Mg2+ concentration of 2·5 mm, 0·5 U Taq DNA polymerase (Qiagen, Hilden, Germany) and 1 × the reaction buffer supplied with the Taq polymerase. The amplification profile consisted of 2 min at 94 °C, followed by 35 cycles consisting of 30 s at 94 °C, 30 s at 60 °C and 30 s at 72 °C, followed by a final extension step of 5 min at 72 °C. The amplifications were carried out in S1000 thermal cyclers (Bio-Rad, Hercules, CA, USA).
A 0·7-μl aliquot of each amplicon was mixed with 7 µl of loading dye (98% formamide, 10 mm EDTA, 0·025% bromophenol blue, 0·025% xylene-cyanol). Following denaturation at 95 °C for 5 min, the samples were place in wet ice and immediately loaded onto 12% acrylamide: bisacrylamide (37·5:1; Bio-Rad) gels (16 cm × 18 cm). Electrophoresis for 18 h in 0·5 × TBE buffer at 200 V was undertaken in Bio-Rad Protean II xi cells with water circulation at 25 °C. The gels were silver-stained using the method of Byun et al. (Reference Byun, Fang, Zhou and Hickford2009).
Sequencing and sequence analysis
PCR amplicons representing different SSCP banding patterns were sequenced in both directions at the Lincoln University DNA Sequencing Facility, NZ. The alignment of sequences, their translation and comparisons between these sequences were carried out using DNAMAN software (version 5.2.10, Lynnon BioSoft, Vaudreuil, Canada).
Statistical analyses
The statistical analyses were performed using SPSS (version 22; IBM, NY, USA). General Linear Models (GLMs) were used to assess the effect of the presence or absence of a particular variant on MY, FP and PP. GLMs were also used to compare variation in MY, FP and PP between different genotypes, with a Bonferroni correction being applied to reduce the chances of obtaining false-positive results during multiple comparisons.
‘Cow age’ (in years) and ‘days in milk’ (counted from the day of calving) affected the milk traits, and thus were included in the models.
We were unable to factor ‘sire’ into the GLMs, as the majority of cows were of unknown paternity because sire genetics (semen straws) were purchased from a commercial semen producer on the basis of quantitative genetic evaluation of performance for key dairy traits. These straws often contain mixed semen, so individual sire identity is impossible to ascertain without access to all the seed stock. However, this weakness can be partially off-set in two ways. Firstly, the cows studied ranged in age between three and nine years and it is unlikely that the same sires were used in the production of mixed semen straws over this period. Secondly, if we concede that cows of the same age may share paternity, the inclusion of ‘cow age’ in the GLMs as an explanatory variable, will at least partially accommodate this effect.
Results and discussion
TLR4 variation in New Zealand dairy cows
Two PCR-SSCP patterns (named A and B) were observed for TLR4 in the cows investigated (Supplementary Fig. S1) and analyses using different SSCP run temperatures for the electrophoresis, did not revealed any further banding patterns. Sequencing of amplicons representative of patterns A and B revealed one SNP (c.2021C/T; rs8193069). This has been previously reported and would result in an amino acid change p.Thr674Ile in the transmembrane/cytoplasmic domain of TLR4 (White et al. Reference White, Taylor, Abbey, Gill and Womack2003). The TLR4 variation observed was considerably less than that reported elsewhere, with White et al. (Reference White, Taylor, Abbey, Gill and Womack2003) reporting 11 SNPs and nine predicted haplotypes for the same bovine gene region. This would suggest there is relatively little genetic variation in TLR4 in NZ HF × J cows and that there has possibly been selective pressure exerted on the gene, and/or some other effect that has reduced genetic diversity.
Three genotypes were detected: AA (n = 141), AB (n = 195) and BB (n = 66), giving frequencies of 59·3% and 40·7% for A and B, respectively. The variants were in Hardy-Weinberg equilibrium (P = 0·918).
Effect of variation in TLR4 on milk traits
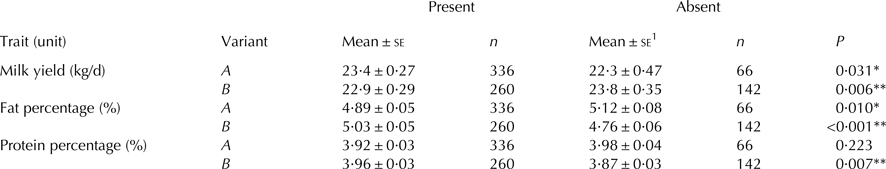
The presence of A was associated with increased MY and decreased FP, whereas B was associated with a decrease in MY and an increase in FP and PP (Table 1). Genotypes were also found to have an effect on MY (P = 0·021) and FP (P < 0·001). AA cows produced more milk than AB or BB cows (AA: 23·9 ± 0·35 kg/d vs AB: 22·9 ± 0·32 kg/d or BB: 22·3 ± 0·47 kg/d). Milk from AA cows had lower FP than milk from AB or BB cows (AA: 4·76 ± 0·06% vs AB: 5·00 ± 0·06% or BB: 5·11 ± 0·08%). A tendency for association was also detected between genotype and PP (P = 0·078).
Association of presence or absence of TLR4 variants with milk production traits

1 Predicted means and standard errors from GLMs. *P < 0·05; **P < 0·01.
The finding that B was associated with increased milk fat and protein percentage, and decreased milk yield; is consistent with the report of Beecher et al. (Reference Beecher, Daly, Childs, Berry, Magee, McCarthy and Giblin2010). However, some differences occur between our findings and those of Beecher et al. (Reference Beecher, Daly, Childs, Berry, Magee, McCarthy and Giblin2010). For example, the effect of variation on milk fat and protein percentage they described was only observed in late lactation, and not in either early or mid-lactation. In our study, this effect was observed across the mid- to late-lactation period. Beecher et al. (Reference Beecher, Daly, Childs, Berry, Magee, McCarthy and Giblin2010) did not report an effect of c.2021C/T on milk yield, as reported here.
The high frequency of B in the NZ cows is consistent with the objectives of the NZ dairy industry's Breeding Worth (BW) system (www.dairynz.co.nz/animal/animal-evaluation/about-nzael/). This breeding system uses an index comprised of eight key dairy traits. It places positive economic value on milk fat and protein percentage, but negative value on milk yield. The negative rating for milk yield is only lightly weighted in the index. In the context of this, B (c.2021T) of TLR4 appears to be a favourable variant for milk production. However, caution would be needed if breeding for this variant, as Sharma et al. (Reference Sharma, Leyva, Schenkel and Karrow2006) reported a lower lactation persistency and a higher somatic cell score (indicative of high susceptibility to mastitis) associated with c.2021T in the daughters of 388 Canadian Holstein bulls. It should be noted that c.2021T was found at a low frequency in these Holstein cattle (Sharma et al. Reference Sharma, Leyva, Schenkel and Karrow2006, Reference Sharma, Abo-Ismail, Schenkel, You, Verschoor, Pant and Karrow2015). Sharma et al. (Reference Sharma, Abo-Ismail, Schenkel, You, Verschoor, Pant and Karrow2015) suggested that c.2021T may affect TLR4 signalling and lead to inadequate induction of immune response genes, and therefore that it may have been selected against by natural selection.
Despite there being a number of studies investigating variation in bovine TLR4 and the relationship of this to susceptibility to mastitis and infectious diseases (Sharma et al. Reference Sharma, Leyva, Schenkel and Karrow2006, Reference Sharma, Abo-Ismail, Schenkel, You, Verschoor, Pant and Karrow2015), little investigation has been undertaken of the c.2021C/T SNP as a consequence of its typically low frequency in the cattle populations investigated. Accordingly further investigation of cattle that have c.2021T is required to ascertain if it does affect immune response.
Supplementary material
The supplementary material for this article can be found at https://doi.org/10.1017/S0022029917000711.
Financial support from the NZ Ministry of Science and Innovation (DRCX 0802) and Lincoln University Gene-Marker Laboratory are acknowledged. We acknowledge the support of AGMARDT for Long Cheng, and thank Innocent Rugoho, Helen Hague, Thomas Vazhathara and Freeman Fang for technical support. We thank Peter Hancox from the Lincoln University Dairy Farm for assistance with sampling.