


INTRODUCTION
Malaria is one of the most important infectious diseases affecting humans, particularly in developing countries. Plasmodium falciparum, an apicomplexan protozoan parasite, is the causative agent of the most lethal form of human malaria. The presence of widespread drug resistance and the lack of a proven vaccine complicate the problem, and limit the available options for effective malaria control. New anti-malarial drugs that interfere with parasite growth are urgently needed, and their rational design and development require the identification of potential therapeutic targets (Renslo and McKerrow, Reference Renslo and McKerrow2006). Detailed knowledge of the molecular mechanisms that control the life cycle of malaria parasites may provide useful information for this purpose (Doerig et al. Reference Doerig, Billker, Haystead, Sharma, Tobin and Waters2008, Reference Doerig, Baker, Billker, Blackman, Chitnis, Dhar Kumar, Heussler, Holder, Kocken, Krishna, Langsley, Lasonder, Menard, Meissner, Pradel, Ranford-Cartwright, Sharma, Sharma, Tardieux, Tatu and Alano2009).
Malaria parasites have a complex life cycle. Infection of humans by P. falciparum, the species responsible for the lethal form of human malaria, begins with the bite of an infected Anopheles mosquito, which delivers sporozoites to the bloodstream. These cells rapidly gain access to the liver and invade hepatocytes, where they undergo substantial multiplication, generating several thousand merozoites (exo-erythrocytic schizogony). The merozoites invade red blood cells (erythrocytic schizogony), the process responsible for malaria pathogenesis. Some merozoites, however, arrest the cell cycle and differentiate into male or female gametocytes, which are infective to the mosquito. Only after being ingested by the insect, the gametocytes develop into gametes and fuse into a zygote (the only diploid stage). Further development in the mosquito involves a process of sporogony, producing sporozoites that accumulate in the salivary glands and are now ready to infect a new human host. The life cycle of malaria parasites is therefore composed of a succession of developmental stages that vary in their proliferative state (massive cell multiplication during schizogony and sporogony, and cell cycle arrest in sporozoites and gametocytes). These different parasite developmental stages require a high degree of adaptation and strict control of the cellular machinery as well as the coordinated modulation of distinct sets of genes. Plasmodium cells regulate these processes by several means, including phosphorylation, transcriptional control, post-transcriptional control and protein degradation. These mechanisms probably involve various interactions between parasite and host signalling molecules and may thus represent strategic targets in the fight against malaria (Doerig et al. Reference Doerig, Baker, Billker, Blackman, Chitnis, Dhar Kumar, Heussler, Holder, Kocken, Krishna, Langsley, Lasonder, Menard, Meissner, Pradel, Ranford-Cartwright, Sharma, Sharma, Tardieux, Tatu and Alano2009).
The modulation of protein phosphorylation through the antagonistic effects of protein kinases and phosphatases is a major regulatory mechanism of many eukaryotic intracellular processes (Manning et al. Reference Manning, Plowman, Hunter and Sudarsanam2002a). The published P. falciparum genome sequence and previous studies have revealed that several homologues of eukaryotic signalling proteins are conserved in P. falciparum (Gardner et al. Reference Gardner, Hall, Fung, White, Berriman, Hyman, Carlton, Pain, Nelson, Bowman, Paulsen, James, Eisen, Rutherford, Salzberg, Craig, Kyes, Chan, Nene, Shallom, Suh, Peterson, Angiuoli, Pertea, Allen, Selengut, Haft, Mather, Vaidya, Martin, Fairlamb, Fraunholz, Roos, Ralph, McFadden, Cummings, Subramanian, Mungall, Venter, Carucci, Hoffman, Newbold, Davis, Fraser and Barrell2002; Chung et al. Reference Chung, Ponts, Cervantes and Le Roch2009; Koyama et al. Reference Koyama, Chakrabarti and Garcia2009), but many of these major mediators have not been characterized for malaria parasites. There is now evidence that protein kinases are essential for the control of the parasite life cycle and that inhibition of such activities can have anti-malarial effects (Doerig et al. Reference Doerig, Abdi, Bland, Eschenlauer, Dorin-Semblat, Fennell, Halbert, Holland, Nivez, Semblat, Sicard and Reininger2010). Moreover, these enzymes are widely recognized as valuable drug targets for the treatment of several diseases (Johnson, Reference Johnson2007; Grant, Reference Grant2009). Analyses of the P. falciparum kinome have revealed 86 or 99 genes (depending on the study) that encode proteins containing kinase domains; however, their functions, mechanisms of regulation and cellular targets are largely unknown (Ward et al. Reference Ward, Equinet, Packer and Doerig2004; Anamika et al. Reference Anamika, Srinivasan and Krupa2005).
cAMP-dependent protein kinase (protein kinase A, or PKA) is a key signal transduction element in mammalian cells, and the regulatory mechanisms of the cAMP pathway are well known (Taylor et al. Reference Taylor, Kim, Cheng, Brown, Wu and Kannan2008b). However, in P. falciparum, components of the cAMP pathway and the precise function of PKA, its downstream target, have not been clearly defined. The cAMP/PKA signalling pathway has attracted interest from a number of research groups, and there are reports of cAMP-dependent protein kinase homologues (PfPKA) in the P. falciparum genome (Li and Cox, Reference Li and Cox2000; Syin et al. Reference Syin, Parzy, Traincard, Boccaccio, Joshi, Lin, Yang, Assemat, Doerig and Langsley2001; Beraldo et al. Reference Beraldo, Almeida, da Silva and Garcia2005; Doerig et al. Reference Doerig, Billker, Haystead, Sharma, Tobin and Waters2008; Merckx et al. Reference Merckx, Echalier, Langford, Sicard, Langsley, Joore, Doerig, Noble and Endicott2008a; Wurtz et al. Reference Wurtz, Pastorino, Almeras, Briolant, Villard and Parzy2009b). The aim of this review is to provide a synthesis of the recent published experimental data on the cAMP/PfPKA signalling pathway, which appears to be essential for parasite growth and survival and, consequently, represents an attractive target for the development of new anti-malarial drugs.
OVERVIEW OF THE cAMP/PKA SIGNALLING PATHWAY
PKA is the best-studied protein kinase, belonging to the AGC group within the eukaryotic protein kinase superfamily (Manning et al. Reference Manning, Plowman, Hunter and Sudarsanam2002a, Reference Manning, Whyte, Martinez, Hunter and Sudarsanamb). It was one of the first protein kinases to be discovered, sequenced and cloned, and the resolution of its structure provided the first three-dimensional template for this family (Walsh et al. Reference Walsh, Perkins and Krebs1968; Shoji et al. Reference Shoji, Parmelee, Wade, Kumar, Ericsson, Walsh, Neurath, Long, Demaille, Fischer and Titani1981; Uhler et al. Reference Uhler, Carmichael, Lee, Chrivia, Krebs and McKnight1986; Knighton et al. Reference Knighton, Zheng, Ten Eyck, Ashford, Xuong, Taylor and Sowadski1991). PKA and cAMP pathways have been implicated in numerous cellular processes, including modulation of other protein kinases, regulation of intracellular calcium concentration and regulation of transcription (Shabb, Reference Shabb2001; Tasken and Aandahl, Reference Tasken and Aandahl2004).
In most organisms, PKA is a heterotetramer composed of 2 regulatory subunits (PKAr), which bind to and inhibit 2 catalytic subunits (PKAc). The cAMP pathway is activated by the binding of a ligand to a membrane-bound G-protein-coupled receptor (GPCR) (7 transmembrane receptor), which interacts with heterotrimeric G-proteins composed of α, β and γ subunits that are bound in the inactive state. The agonist binding triggers a conformational change in the receptor, which catalyses the exchange from GDP to GTP and the dissociation of Gα from Gβγ subunits. Both Gα and Gβγ subunits can modulate the activity of downstream effectors. In particular, Gα subunit proteins are divided into 4 subfamilies (Gαs, Gαi, Gαq and Gα12/13) (Hamm, Reference Hamm1998) and a single GPCR can couple to 1 or more families resulting in different cellular responses (Cabrera-Vera et al. Reference Cabrera-Vera, Vanhauwe, Thomas, Medkova, Preininger, Mazzoni and Hamm2003). When coupling to Gαs or Gαi proteins, GPCRs either activate or inhibit adenylate cyclase (AC) activity resulting in an increase or decrease in cAMP formation, respectively (Cabrera-Vera et al. Reference Cabrera-Vera, Vanhauwe, Thomas, Medkova, Preininger, Mazzoni and Hamm2003). The flux through the pathway is controlled by the self-inactivating GTPase activity of the Gα subunit, which hydrolyses GTP to GDP, resulting in reassociation of the Gα subunit with the Gβγ subunits and termination of the G protein signalling. The binding of 2 cAMP molecules to each PKAr alters its affinity for the catalytic subunit, resulting in release of the active PKAc. PKAc, a serine/threonine kinase, can phosphorylate many substrates, such as additional protein kinases and transcription factors (Shabb, Reference Shabb2001). The termination of cAMP signalling is conferred by a large superfamily of enzymes known as phosphodiesterase proteins (PDE) that catalyse the degradation of cAMP into 5′AMP (Fimia and Sassone-Corsi, Reference Fimia and Sassone-Corsi2001; Lugnier, Reference Lugnier2006). The intracellular concentrations of cAMP are therefore regulated by the counterbalancing activities of ACs and PDEs. In addition, the signalling events induced by agonist activation of GPCRs can be counteracted in the cell by intrinsic mechanisms known as the receptor desensitization. Phosphorylation is the most rapid means of GPCR desensitization and is achieved by 2 classes of serine/threonine protein kinases: PKAc directly via a feedback regulation and G protein-coupled receptor kinases (GRKs). GRK-mediated receptor phosphorylation promotes the binding of β-arrestins, which not only uncouple receptors from heterotrimeric G proteins but also target many GPCRs for internalization, followed by either recycling or degradation of the receptor (Lefkowitz, Reference Lefkowitz1998; Ferguson, Reference Ferguson2001; Hendriks-Balk et al. Reference Hendriks-Balk, Peters, Michel and Alewijnse2008). In mammalian cells, PKA contains 3 catalytic subunit isoforms (Cα, Cβ and Cγ) and 4 regulatory subunit isoforms (RIα, RIβ, RIIα and RIIβ) (Doskeland et al. Reference Doskeland, Maronde and Gjertsen1993). The tissue-specific expression and assembly patterns of these kinase isoforms are thought to be responsible for the diverse cellular responses to cAMP (Taylor et al. Reference Taylor, Buechler and Yonemoto1990). PKAc activity can be regulated by binding to protein kinase inhibitor (PKI), its natural endogenous inhibitor (Dalton and Dewey, Reference Dalton and Dewey2006). PKI inhibits the activity of PKAc by binding to free catalytic subunits of this enzyme and inhibiting the phosphorylation of PKAc substrates (Ashby and Walsh, Reference Ashby and Walsh1972, Reference Ashby and Walsh1973). PKI is similar to the PKAr in that both proteins contain amino acid sequences (pseudosubstrate sites) that allow them to bind to the PKAc and inhibit its activity. The functional specificity of PKA is largely dependent on the targeting of the catalytic subunit to specific substrates at precise locations in the cell. This is accomplished by the A-kinase anchoring-protein (AKAP) family, whose members are bound to subcellular structures and recruit PKA via interactions with the regulatory subunit (Barradeau et al. Reference Barradeau, Imaizumi-Scherrer, Weiss and Faust2002; McConnachie et al. Reference McConnachie, Langeberg and Scott2006).
P. falciparum cAMP-dependent protein kinase activity has been detected in cytosolic extracts of both the asexual and sexual stages of the parasite, and a putative regulatory subunit has been identified in asexual forms (Kaushal et al. Reference Kaushal, Carter, Miller and Krishna1980; Read and Mikkelsen, Reference Read and Mikkelsen1990; Read and Mikkelsen, Reference Read and Mikkelsen1991b), suggesting the existence of the cAMP pathway in the parasite (Fig. 1). The single P. falciparum PKA catalytic subunit (pfpkac) gene was first isolated and characterized using a PCR-based approach, which identified a DNA fragment that shared high sequence homology with catalytic subunits of the PKA family (Li and Cox, Reference Li and Cox2000). Subsequent studies of this kinase have illuminated much about its structure and substrate specificity (Syin et al. Reference Syin, Parzy, Traincard, Boccaccio, Joshi, Lin, Yang, Assemat, Doerig and Langsley2001; Sudo et al. Reference Sudo, Kato, Kobayashi, Tohya and Akashi2008; Wurtz et al. Reference Wurtz, Pastorino, Almeras, Briolant, Villard and Parzy2009b).
Schematic model of cAMP/PKA signalling pathway in Plasmodium falciparum. This pathway is based on data reported in the literature. All elements that are not known or not proven are associated with a question mark. The pathway begins when an unknown ligand activates a GPCR. The transduction signal is transmitted to G-proteins (not yet identified in P. falciparum), which activate adenylate cyclase. The latter allows the production of cAMP from ATP. The cAMP binds to the PfPKAr, which changes its conformation and allows the release of PfPKAc. Once free, PfPKAc phosphorylates unknown substrates using ATP as the phosphate donor. PDEs degrade cAMP and thus limit PfPKAc activation. In P. falciparum, the existence of AKAP proteins has not yet been proven, but an orthologue of P. yoelli AKAP is annotated in the P. falciparum genome as a conserved protein with unknown function (PFE0640w). The signalling events induced by agonist activation of GPCRs can be counteracted in eukaryotes by PKAc directly or by GRKs. However, in Plasmodium these mechanisms, as well as GRKs, have not been identified.

The single P. falciparum PKA regulatory subunit (PfPKAr) was first identified using BLASTP analyses (Altschul et al. Reference Altschul, Gish, Miller, Myers and Lipman1990) with PKAr subunits from various eukaryotes as queries, and the gene was later cloned and expressed (Ward et al. Reference Ward, Equinet, Packer and Doerig2004; Merckx et al. Reference Merckx, Nivez, Bouyer, Alano, Langsley, Deitsch, Thomas, Doerig and Egee2008b).
An AC activity, biochemically distinct from that of the host was first measured in P. falciparum by Mikkelsen and Read (Read and Mikkelsen, Reference Read and Mikkelsen1991b). Two different genes with high homology to ACs (PfACα PF14_0788 and PfACβ MAL8P1.150) have been identified and characterized in P. falciparum (Muhia et al. Reference Muhia, Swales, Eckstein-Ludwig, Saran, Polley, Kelly, Schaap, Krishna and Baker2003; Baker, Reference Baker2004; Baker and Kelly, Reference Baker and Kelly2004; Weber et al. Reference Weber, Vishnyakov, Hambach, Schultz, Schultz and Linder2004). Four putative P. falciparum PDEs have now been identified, containing the class I signature motif and sharing approximately 40% amino acid identity (PfPDEα PFL0475w, PfPDEβ MAL13P1.118, PfPDEγ MAL13P1.119 and PfPDEδ PF14_0672). The cyclic nucleotide specificity of the 4 encoded enzymes cannot be predicted on the basis of primary amino acid sequence, but it seems that PfPDEα and PfPDEδ are more specific to cGMP (Yuasa et al. Reference Yuasa, Mi-Ichi, Kobayashi, Yamanouchi, Kotera, Kita and Omori2005; Taylor et al. Reference Taylor, McRobert and Baker2008a; Wentzinger et al. Reference Wentzinger, Bopp, Tenor, Klar, Brun, Beck and Seebeck2008). In the PlasmoDB database, 2 genes coding for a G-protein coupled receptor, putative (PFE1265w) and for a G-protein associated signal transduction protein, putative (PFF0365c) have been found, but no other data are available regarding the function of these two proteins. In addition, Madeira and coworkers have identified 4 putative serpentine receptors in P. falciparum (PF11_0321, PFL0765w, PFD1075w, MAL7P1.64), but again, their roles and their implication in the cAMP pathway have not been defined (Madeira et al. Reference Madeira, Galante, Budu, Azevedo, Malnic and Garcia2008). They predicted that these receptors could be implicated in sensing extracellular signal and that elucidation of their detailed function may highlight the mechanisms used by the parasite to modulate its life cycle. Results consistent with the presence of heterotrimeric G proteins in P. falciparum have also been reported, and it has been suggested that they might be involved in the switch to sexual development (Dyer and Day, Reference Dyer and Day2000). However, until now no gene encoding heterotrimeric G-proteins have been identified in P. falciparum genome. On the other hand, it has recently been proposed that the cAMP signalling system of the red blood cell could play a role in malaria infection (Harrison et al. Reference Harrison, Samuel, Akompong, Hamm, Mohandas, Lomasney and Haldar2003). Indeed, host GPCRs and Gαs appear to be associated with the parasite vacuole (Lauer et al. Reference Lauer, VanWye, Harrison, McManus, Samuel, Hiller, Mohandas and Haldar2000) and addition of peptides that block the interaction between GPCR and Gαs led to decreased parasitaemia (Harrison et al. Reference Harrison, Samuel, Akompong, Hamm, Mohandas, Lomasney and Haldar2003). Finally, until now, only 1 AKAP was annotated in the P. yoelii genome (PY04627) (Carlton et al. Reference Carlton, Angiuoli, Suh, Kooij, Pertea, Silva, Ermolaeva, Allen, Selengut, Koo, Peterson, Pop, Kosack, Shumway, Bidwell, Shallom, van Aken, Riedmuller, Feldblyum, Cho, Quackenbush, Sedegah, Shoaibi, Cummings, Florens, Yates, Raine, Sinden, Harris, Cunningham, Preiser, Bergman, Vaidya, van Lin, Janse, Waters, Smith, White, Salzberg, Venter, Fraser, Hoffman, Gardner and Carucci2002). In P. falciparum, an orthologue of this AKAP has been annotated as a conserved protein with unknown function (PFE0640w), but no study has been conducted on this topic.
The knowledge of signal-transduction pathways in Plasmodium is fundamental to allow the design of new strategies against malaria. According to these previous data, there is evidence that the cAMP/PKA pathway exists in the malaria parasite. However, a number of important components in this pathway have so far not yet been clearly defined and must be studied more thoroughly: the ligand-receptor complex that initiates the cAMP pathway (GPCRs), the signalling molecules that activate AC (is this mediated by heterotrimeric G proteins in P. falciparum or not?), the regulation of this cellular network (do GRK, PKI and feedback PKAc control the mechanisms of regulation in the parasite?), and the downstream targets of PfPKAc.
STRUCTURE OF THE cAMP-DEPENDENT PROTEIN KINASE COMPLEX
cAMP-dependent protein kinase catalytic subunit
The PFI1685w gene in the PlasmoDB database (Bahl et al. Reference Bahl, Brunk, Crabtree, Fraunholz, Gajria, Grant, Ginsburg, Gupta, Kissinger, Labo, Li, Mailman, Milgram, Pearson, Roos, Schug, Stoeckert and Whetzel2003) has 4 introns and 5 exons, and the protein product, PfPKAc, has a predicted molecular mass of 40·2 kDa and a calculated pI of 9·11. Comparative analyses using BLASTP revealed that the amino acid sequence of PfPKAc shares about 50% of identity with PKAc from Homo sapiens and Mus musculus and high homology (88%) with P. yoelii PKAc (http://blast.ncbi.nlm.nih.gov/Blast.cgi). A multiple sequence alignment of the amino acid sequences of PKAc from various organisms using T-Coffee method (Notredame et al. Reference Notredame, Higgins and Heringa2000; Poirot et al. Reference Poirot, O'Toole and Notredame2003) showed strong conservation of the 11 specific kinase subdomains (I-XI) among the different organisms. Several residues required for catalytic activity are also highly conserved (Hanks et al. Reference Hanks, Quinn and Hunter1988) (Fig. 2A and B and Table 1). A three-dimensional model of PfPKAc was created based on the crystal structure of Homo sapiens PKAc alpha subunit (HsPKAc; PDB accession number 2GU8) using the Swiss-Model ternary structure prediction tool (Arnold et al. Reference Arnold, Bordoli, Kopp and Schwede2006) and Pymol 0.99 software (DeLano, Reference DeLano2008) (Fig. 2B). As expected, and due to a high degree of primary sequence similarity (50% identity) between the two proteins, the PfPKAc model showed structural homology to HsPKAc. The PKAc subunits are bilobal enzymes with 2 major domains (the small N-terminal lobe and the large C-terminal lobe) that are conserved throughout the protein kinase family (Hanks et al. Reference Hanks, Quinn and Hunter1988; Taylor et al. Reference Taylor, Buechler and Yonemoto1990; Hanks and Hunter, Reference Hanks and Hunter1995; Smith et al. Reference Smith, Radzio-Andzelm, Madhusudan, Akamine and Taylor1999; Johnson et al. Reference Johnson, Akamine, Radzio-Andzelm, Madhusudan and Taylor2001; Taylor et al. Reference Taylor, Kim, Cheng, Brown, Wu and Kannan2008b). The smaller N-terminal lobe, which includes subdomains I–IV, is primarily involved in the anchoring and orientation of ATP. This lobe has a predominantly anti-parallel β-sheet structure. The larger C-terminal lobe, which comprises subdomains VI to XI, is mainly composed of α-helices. It serves as a framework for the catalytic machinery and also as a docking scaffold for binding to protein partners that act as substrates or inhibitors. Moreover, the N-terminal lobe can also be involved in docking with some proteins and partners, for example, the A Kinase Interacting Protein (AKIP 1) binds to the N-terminus of PKAc and helps to traffic it into the nucleus (Sastri et al. Reference Sastri, Barraclough, Carmichael and Taylor2005; Taylor et al. Reference Taylor, Kim, Cheng, Brown, Wu and Kannan2008b; Kornev and Taylor, Reference Kornev and Taylor2010). Table 1 summarizes the important residues, secondary structure and function of each subdomain for both HsPKAc and PfPKAc. We are particularly interested in the sequence and structural differences between HsPKAc and PfPKAc, as the ultimate goal of this study is to design molecules that specifically target the parasite enzyme (Fig. 2B and Table 1). The first divergence concerns subdomain I, which is composed of 2 β-strands and 2 α-helices in PfPKAc but consists of 2 β-strands only in HsPKAc. As shown in Table 1, this subdomain participates in ATP anchoring. Next, in subdomain VI, a β-strand and an α-helix are missing from the PfPKAc model. This domain contains the putative catalytic loop sequence HRDLKXXN, which includes an aspartate identified as the candidate catalytic base (Hanks and Hunter, Reference Hanks and Hunter1995). The last notable divergence concerns subdomain VIII, where the α-helix in HsPKAc is divided into 2 α-helices in PfPKAc. In the same domain, a β-strand was also absent in PfPKAc model as compared to the HsPKAc structure. Moreover, a tryptophan (W196) previously identified as essential for mammalian PKAr binding is not conserved in the PfPKAc subdomain VIII sequence (Y187) (Gibson and Taylor, Reference Gibson and Taylor1997; Kim et al. Reference Kim, Xuong and Taylor2005). Other differences between PfPKAc and HsPKAc were also observed, but these were not located in known functional domains (Table 1).
Amino acid sequence alignments and structural modelling of PfPKAc. (A) Comparison of the PfPKAc amino acid sequence with those of other protein kinase catalytic subunits. Plasmodium falciparum (Uniprot Accession number Q7K6A0), Homo sapiens (P17612), Mus musculus (P05132), Plasmodium yoelii (Q7RE33), Cryptosporidium parvum (A3FQ39), Trypanosoma brucei (Q38DR5), Saccharomyces cerevisae (P06244) and Drosophila melanogaster (P12370) were aligned using T-coffee 7.38 and CLUSTAL format. The 11 typical subdomains are indicated with boxed regions and Roman numerals. Identical residues (asterisks), conservative substitutions (colons) and semi-conservative substitutions (dots) are also indicated. (B) Structural model of PfPKAc. The PfPKAc structure was modelled on the resolved structure of human PKAc alpha. The different colours represent the 11 subdomains characteristic of protein kinases. The small N-terminal lobe, which is involved in ATP binding, and the large C-terminal lobe, which comprises the catalytic regions and substrate-binding domain, are represented in the figure. α-helices (cylinders), β-sheets (arrows) and turns (lines) are indicated, as are secondary structure differences in PfPKAc (purple) and essential residues in both structures (red dots).

Major structural features of the catalytic domain of PKAc from Homo sapiens and Plasmodium falciparum

ND, Not determined.
Despite its high sequence identity and strong structural homology with HsPKAc, PfPKAc presents some interesting differences in essential domains involved in the following functions: (i) ATP anchoring, (ii) mechanisms of substrate phosphorylation and (iii) substrate recognition and/or inhibitor sensitivity. The development of new anti-malarial compounds targeting these domains could allow for the inhibition of the parasite enzyme with low levels of host protein interaction.
cAMP-dependent protein kinase regulatory subunit
The PFL1110c gene in the PlasmoDB database has 2 introns and 3 exons, and the protein product, PfPKAr, has a predicted molecular mass of 50·8 kDa and a calculated pI of 7·49. Comparative analyses using BLASTP revealed that the amino acid sequence of PfPKAr shares ∼41% identity with PKAr from Homo sapiens, Bos taurus and Mus musculus and high homology with P. knowlesi strain H PKAr (73%) (http://blast.ncbi.nlm.nih.gov/Blast.cgi). A multiple sequence alignment of the amino acid sequences of PKAr from various organisms using the T-coffee program (Notredame et al. Reference Notredame, Higgins and Heringa2000; Poirot et al. Reference Poirot, O'Toole and Notredame2003) revealed a similar general architectural organization among the various organisms and several residues required for regulatory activity, as well as some interesting differences (Taylor et al. Reference Taylor, Buechler and Yonemoto1990) (Fig. 3A and B and Table 2). The nuclear magnetic resonance (NMR) structures of mammalian type I and type II regulatory subunit D/D domains have been solved (Banky et al. Reference Banky, Huang and Taylor1998; Newlon et al. Reference Newlon, Roy, Morikis, Carr, Westphal, Scott and Jennings2001), as have the crystal structures of the isolated CBD-A and CBD-B (Diller et al. Reference Diller, Madhusudan, Xuong and Taylor2001; Su et al. Reference Su, Dostmann, Herberg, Durick, Xuong, Ten Eyck, Taylor and Varughese1995). However, no high-resolution structures are available for the full-length regulatory subunit, linker regions or cAMP-free regulatory subunits. Thus, we created a three-dimensional model of PfPKAr based on the crystal structure of a 1–91 deletion mutant of the type I alpha regulatory subunit from B. taurus (BtPKAr; PDB Accession number 1RGS) using the Swiss-Model ternary structure prediction tool and Pymol software. The BtPKAr sequence is very close to that of H. sapiens PKAr (97% identity), which does not have a described structure.
Amino acid sequence alignments and partial structural modelling of PfPKAr. (A) Comparison of PfPKAr amino acid sequence with other protein kinase regulatory subunits. Plasmodium falciparum (Uniprot Accession number Q7KQK0), H. sapiens (P10644), B. taurus (P00514), M. musculus (Q9DBC7), C. parvum (A3FPL6), T. brucei (Q9GU80), S. cerevisae (P07278), P. knowlesi (B3LCL9) and D. melanogaster (Q9VPA) were aligned using T-coffee 7.38 and CLUSTAL format. The AKAP binding and dimerization domain, inhibitory sequence and cAMP-binding domains A and B are indicated (black boxed regions). Phosphate-binding cassettes A and B (red rectangles), β-sheets (yellow) and α-helixes (turquoise blue) are depicted as in Fig. 2B. Secondary structural element differences between B. taurus PKAr and PfPKAr are shown in purple. Identical residues (asterisks), conservative (colons) and semi-conservative substitutions (dots) are also indicated. (B) Structural model of partial PfPKAr. The partial PfPKAr structure was modelled on the resolved structure of B. taurus 1-91 deletion mutant type I alpha PKAr. α-helices (blue cylinders), β-sheets (yellow arrows) and turns (lines) are illustrated. Secondary structural differences between PfPKAr and PfPKAc are shown in purple. Phosphate-binding cassettes A and B are shown in red.

Major structural features of the regulatory domain of PKAr from Bos taurus and Plasmodium falciparum
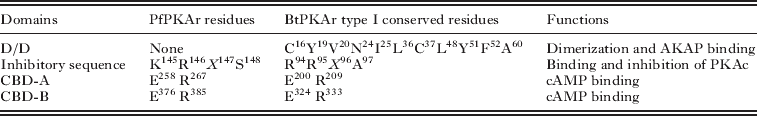
D/D, Dimerization/docking domain.
CBD, cAMP-binding domain.
In most cells, the regulatory subunit is typically a highly asymmetric dimer composed of different domains. The amino-terminal region of the regulatory subunit (1–140) corresponds to the dimerization/docking domain (D/D) responsible for homodimerization. Once dimerized, this region also provides a binding surface for the AKAPs (Banky et al. Reference Banky, Huang and Taylor1998; Newlon et al. Reference Newlon, Roy, Morikis, Carr, Westphal, Scott and Jennings2001). The D/D domain of the type I regulatory subunit contains a number of conserved residues that are critical for dimerization and AKAP binding (C16, Y19, V20, N24, I25, L36, C37, L48, Y51, F52 and A60 in BtPKAr) (Leon et al. Reference Leon, Herberg, Banky and Taylor1997; Gibson et al. Reference Gibson, Schanen, Chakrabarti and Chakrabarti2006) (Fig. 3A and Table 2). This N-terminal sequence, which encodes the regulatory D/D domain found in most regulatory subunits, is not present in the parasite protein, suggesting that it does not undergo regulatory subunit dimer formation as previously reported for P. falciparum (Syin et al. Reference Syin, Parzy, Traincard, Boccaccio, Joshi, Lin, Yang, Assemat, Doerig and Langsley2001; Merckx et al. Reference Merckx, Nivez, Bouyer, Alano, Langsley, Deitsch, Thomas, Doerig and Egee2008b) and several other organisms (Mutzel et al. Reference Mutzel, Lacombe, Simon, de Gunzburg and Veron1987; Carlson and Nelson, Reference Carlson and Nelson1996). While an orthologue of P. yoelii AKAP is found in P. falciparum genome, no consensus AKAP-binding domain was present in the P. falciparum regulatory subunit. This suggests that the parasite uses a mode of binding between AKAP and PfPKAr that is distinct from that of other species (Barradeau et al. Reference Barradeau, Imaizumi-Scherrer, Weiss and Faust2002; McConnachie et al. Reference McConnachie, Langeberg and Scott2006).
In mammals, the D/D domain is followed by a flexible linker region that contains an inhibitory site. This site, generally located between residues 90 and 100 in the regulatory subunit, binds to and inhibits the active site of the catalytic subunit (Li et al. Reference Li, Gangal, Jones, Deich, Lovett, Taylor and Johnson2000). The amino acid sequence of this region is similar to that of its catalytic subunit substrates and thus can be used to differentiate between type I and type II regulatory subunits. This region includes either a pseudosubstrate site (RRXA or RRXG in type I regulatory subunits) or an autophosphorylation region with a serine at the phosphorylation site (RRXS in type II regulatory subunits) (Taylor et al. Reference Taylor, Buechler and Yonemoto1990). The overall architecture of PfPKAr is closer to type I BtPKAr, but it presents a degenerated inhibitory sequence (KRXS) containing 1 of 2 important arginines and a serine autophosphorylated site similar to that of type II BtPKAr. Thus, PfPKAr seems to share characteristics with both type I and type II BtPKAr.
The C-terminal end of the mammalian regulatory subunit contains 2 tandem cAMP-binding domains (CBDs), named A and B (Takio et al. Reference Takio, Smith, Krebs, Walsh and Titani1984). Binding of cAMP to the CBD of the regulatory subunit dissociates the catalytic subunit, which becomes catalytically active. These CBDs, which probably resulted from domain duplication, show a strong sequence homology among the different organisms. Comparison of PfPKAr with other mammalian PKAr reveals the existence of these two highly conserved CBDs, which contain essential residues necessary for cAMP binding: a conserved glutamate that binds to the 2′OH of the ribose (E200 and E324 in BtCBD-A and BtCBD-B, respectively) and a conserved arginine that interacts with the phosphate of cAMP (R209 and R333 in BtCBD-A and BtCBD-B, respectively) (Taylor et al. Reference Taylor, Buechler and Yonemoto1990; Su et al. Reference Su, Dostmann, Herberg, Durick, Xuong, Ten Eyck, Taylor and Varughese1995; Berman et al. Reference Berman, Ten Eyck, Goodsell, Haste, Kornev and Taylor2005) (Fig. 3A and Table 2). These residues are part of an important motif called the phosphate-binding cassette (PBC) that is present in each of the CBDs (PBC-A and PBC-B). The structure of the truncated PfPKAr revealed strong structural homology with BtPKAr (Fig. 3B). The CBD is a small module, about 120 amino acids in length, which consists of helical domains and an 8-stranded β-barrel where cAMP binds. The essential feature of the β-barrel is the conserved PBC that anchors cAMP and shields it from solvent interactions (Canaves and Taylor, Reference Canaves and Taylor2002). The PBCs comprise β-strand 6, a short turn of α-helix and β-strand 7. Most of the variability in the CBDs corresponds to the loop between β-strand 4 and β-strand 5 and the C-terminal region of each A and B domain. In P. falciparum, the 2 CBDs are well conserved; however, there are slight differences between them, especially in the C-terminal area of each CBD, where the α-helices 7 and 8 present in BtPKAr structure are grouped into a single helix in PfPKAr (Fig. 3B).
Analysis of the amino acid sequence and structure of PfPKAr indicates that it shares a number of conserved features with other PKAr proteins. However, there are also several interesting differences, including the degenerate D/D domain and the inhibitory sequence, which is a mixture between type I and type II regulatory subunits.
PHYLOGENETIC ANALYSIS OF PFPKA
Phylogenetic analyses of PKAc and PKAr were performed with sequences from 18 different species, including representatives of Apicomplexa, Euglenozoa and Metazoa phyla. The results are shown in Fig. 4. The methods used to infer the phylogenetic trees are presented in the legend of the figure. The Metazoa clade is fully supported, with 100% bootstrap values in the phylogenetic analyses of both PKAr and PKAc sequences. Within the Metazoa, mammals (B. taurus, Rattus norvegicus, Mus musculus and H. sapiens) are grouped together (100% bootstrap), and the mammalian relationships are congruent between the two datasets, although with weaker support in the PKAr analysis. Both datasets group the Euglenozoa as a monophyletic clade, with 87% and 100% bootstrap values for PKAc and PKAr, respectively. The Apicomplexa are monophyletic in the PKAr tree and paraphyletic in the PKAc tree. This paraphyly could be explained by the low support for the positions of Apicomplexans Toxoplasma gondii, Cryptosporidium parvum and Babesia bovis and their long respective branches in both analyses. With both genes, the Plasmodium species are grouped in a strongly supported clade (100% bootstrap). The 3 rodent malaria parasites, P. berghei, P. yoelii and P. chabaudi, form a group with a high bootstrap value that is separated from the human malaria species. Concerning the human parasites, P. vivax and P. knowlesi are clustered together but P. falciparum is either at the root of these species (PKAc) or at the root of the rodent ones (PKAr). The P. falciparum branches are the longest among the Plasmodium species. The phylogenetic distance between Plasmodium species and their vertebrate host (H. sapiens) is considerable for both PKAc and PKAr. This information, together with the differences observed in sequences and structures, supports the idea that PfPKA can be specifically inhibited, further establishing this protein as an interesting target for anti-malarial compounds.
Phylogenetic tree of cAMP-dependent protein kinase catalytic (A) and regulatory (B) subunits. The PKA protein sequences of 17 species have been obtained from UniProt Knowledgebase (http://www.ebi.ac.uk/uniprot/): Plasmodium falciparum, P. vivax (Accession number PKAc A5KE97-PKAr A5K031), P. yoelii (PKAr Q7RJ15), P. knowlesi (B3L322-B3LCL9), P. chabaudi (Q4XMV3-Q4Y575), P. berghei (Q4YW20-Q4YNR9), Babesia bovis (A7ANK3-A7AU83), Cryptosporidium parvum, Toxoplasma gondii (B6KN50-Q9BMY7), Trypanosoma brucei, Leishmania major (Q27687-Q4QGD8), Homo sapiens, Mus musculus, Rattus norvegicus (A1L1M0-P09456), Bos taurus (PKAc P00517), Drosophila melanogaster and Caenorhabditis elegans (P21137-P30625). Multiple alignments of these sequences were performed using T-coffee (default parameters) (Notredame et al. Reference Notredame, Higgins and Heringa2000). Selection of the best-fit substitution model was done by a test run with ProTest software on each of the protein alignments (Abascal et al. Reference Abascal, Zardoya and Posada2005). Phylogenetic relationships among sequences were determined using the maximum likelihood (ML) method implemented in PhyML (Guindon and Gascuel, Reference Guindon and Gascuel2003) using the LG+G model. The additional parameters used in PhyML analyses were as follows: gamma distribution parameter estimated with 4 rates categories, and subtree pruning and regrafting (SPR) tree search method from 5 random starting trees (Hordijk and Gascuel, Reference Hordijk and Gascuel2005). Significances of internal branches are indicated as percentages based on 100 bootstrap replications (only bootstrap values >50% are shown). The online tool ‘Interactive Tree Of Life’ was used for the display and manipulation of the phylogenetic trees (Letunic and Bork, Reference Letunic and Bork2007). The phylogenetic analysis included 17 eukaryotes belonging to 3 groups: Metozoa (blue), Euglenozoa (pink) and Apicomplexa (green). The Metazoa group was used as an outgroup in the analyses.

METHODS TO STUDY THE PKA AND CAMP PATHWAY IN P. FALCIPARUM
The biochemical and biological studies of PfPKA has been dominated by the use of either pharmacological inhibitors/activators of members of the cAMP pathway or by molecular strategies.
Biochemical strategies
Two compounds in particular have been widely used to study PKAc function in eukaryotic cells: H89 and KT5720. H89 is an isoquinoline derivative developed from inhibitor H8 (Hidaka et al. Reference Hidaka, Inagaki, Kawamoto and Sasaki1984), while KT5720 belongs to a family of compounds synthesized by the fungus Nocardiopsis sp. (Kase et al. Reference Kase, Iwahashi, Nakanishi, Matsuda, Yamada, Takahashi, Murakata, Sato and Kaneko1987). Both inhibitors act through similar mechanisms as competitive antagonists of ATP at its PKAc binding site, thus preventing cAMP-dependent phosphorylation of PKAc substrates. However, these two compounds seem to have various non-specific effects, such as inhibiting other protein kinases, sometimes more potently than their intended target (Davies et al. Reference Davies, Reddy, Caivano and Cohen2000; Murray, Reference Murray2008).
Rp-cAMP, another PKAc inhibitor, acts as a competitive antagonist of cAMP by binding to PKAr (on CBD domain) without dissociating the kinase holoenzyme (Gjertsen et al. Reference Gjertsen, Mellgren, Otten, Maronde, Genieser, Jastorff, Vintermyr, McKnight and Doskeland1995). In contrast to H89 and KT5720, this compound may not have effects outside the cAMP signalling pathways (Murray, Reference Murray2008).
PKI peptide, which is an endogenous molecule involved in the regulation of PKA activity, binds to free PKAc and prevents the phosphorylation of PKAc targets. PKI seems to be a more specific PKAc inhibitor than H89 or KT5720, but all three have been widely used to study PfPKA and cAMP signalling in P. falciparum. Other inhibitors of the cAMP pathway that specifically target AC, such as MDL-12, SQ22536 and dideoxyadenosine were also used and lead to cAMP depletion, impeding PKAc activation.
Activation of cAMP pathway elements is another way to study the function of PfPKAc and, more generally, the organization of the cAMP pathway in P. falciparum. Different molecules targeting PKAc directly or indirectly can be employed. Forskolin, a labdane diterpene produced by the Coleus forskohlii plant (Takeda et al. Reference Takeda, Adachi, Halprin, Itami, Levine and Woodyard1983), acts by activating the AC enzyme, resulting in an increase of cAMP level and thus allowing PKAc activation. It is interesting to note that AC activity is insensitive to forskolin in asexual blood stages (Read and Mikkelsen, Reference Read and Mikkelsen1991b), while ACα in sporozoites seems to be sensitive to forskolin stimulation (Ono et al. Reference Ono, Cabrita-Santos, Leitao, Bettiol, Purcell, Diaz-Pulido, Andrews, Tadakuma, Bhanot, Mota and Rodriguez2008). Many pathogenic bacteria secrete toxins, such as the cholera and pertussis toxins, that alter the intracellular concentration of cAMP. These toxins disrupt the normal regulation of the cAMP pathway by catalysing the ADP-ribosylation of the heterotrimeric G proteins, which prevents AC inactivation. Thus, AC remains inappropriately active, leading to an increase in cAMP concentration that activates PKAc. Another way to stimulate PKAc activity is to add cAMP analogues such as 8-Br-cAMP or 6-Bz-cAMP directly to the cell. PKAc activity can also be induced by preventing the destruction of cAMP by phosphodiesterases. Some molecules, including IBMX and caffeine, inhibit the action of these enzymes, allowing cAMP to accumulate in the cell thereby leading to the activation of PKAc. It should be noted, however, that these molecules had little or no effect when tested on native PfPDE enzyme activity (McRobert et al. Reference McRobert, Taylor, Deng, Fivelman, Cummings, Polley, Billker and Baker2008), but can be used to clarify and to understand the pathway connections in the parasite.
Molecular strategies
Other molecular techniques have been developed to study the cAMP-signalling pathway, such as RNA interference (RNAi). Briefly, double-stranded RNAs (dsRNA) targeting a specific cellular mRNA can be introduced to the cell to knock down the encoded proteins. To date, RNAi-related genes have not been identified in the P. falciparum genome (Ullu et al. Reference Ullu, Tschudi and Chakraborty2004; Baum et al. Reference Baum, Papenfuss, Mair, Janse, Vlachou, Waters, Cowman, Crabb and de Koning-Ward2009), it has been suggested that the inhibitory effect of dsRNA might be due to an antisense effect rather than a classical RNAi mechanism (McRobert and McConkey, Reference McRobert and McConkey2002; Noonpakdee et al. Reference Noonpakdee, Pothikasikorn, Nimitsantiwong and Wilairat2003; Gunasekera et al. Reference Gunasekera, Patankar, Schug, Eisen, Kissinger, Roos and Wirth2004; Gissot et al. Reference Gissot, Briquet, Refour, Boschet and Vaquero2005; Rathjen et al. Reference Rathjen, Nicol, McConkey and Dalmay2006). Another possibility is that the proteins involved in RNAi processes (Dicer, RNA-Induced Silencing Complex …) could be transported into the parasite from the human host cell (Rathjen et al. Reference Rathjen, Nicol, McConkey and Dalmay2006). Although there has been some controversy surrounding the utility and effectiveness of RNAi in P. falciparum (Ullu et al. Reference Ullu, Tschudi and Chakraborty2004; Baum et al. Reference Baum, Papenfuss, Mair, Janse, Vlachou, Waters, Cowman, Crabb and de Koning-Ward2009), dsRNAs have been employed to explore the biological function of some P. falciparum proteins (Kumar et al. Reference Kumar, Adams, Oldenburg, Musiyenko and Barik2002; Malhotra et al. Reference Malhotra, Dasaradhi, Kumar, Mohmmed, Agrawal, Bhatnagar and Chauhan2002; McRobert and McConkey, Reference McRobert and McConkey2002; Pradhan and Tuteja, Reference Pradhan and Tuteja2007; Sriwilaijaroen et al. Reference Sriwilaijaroen, Boonma, Attasart, Pothikasikorn, Panyim and Noonpakdee2009).
When the level of pfpkac mRNAs is down-regulated using dsRNA, the cAMP pathway is inhibited (Wurtz et al. Reference Wurtz, Desplans and Parzy2009a). Moreover, introduction of a non-functioning mutant or over-expression of some proteins using plasmid transfection can be used to specifically perturb signalling pathways (Merckx et al. Reference Merckx, Nivez, Bouyer, Alano, Langsley, Deitsch, Thomas, Doerig and Egee2008b). The major drawbacks to these strategies are the low transfection efficiencies and the complexity of implementing these techniques (Meissner et al. Reference Meissner, Breinich, Gilson and Crabb2007). However, given the high specificity of such techniques relative to pharmacological agents, it is likely that molecular strategies will further improve the understanding of signalling pathways in Plasmodium.
BIOLOGICAL FUNCTIONS OF PFPKA
While the downstream targets of PfPKAc have not yet been clearly identified, several reports have suggested that this enzyme seems to play a pleiotropic role during the different stages of the parasite life cycle. First, PfPKAc seems to be involved in asexual parasite development, including erythrocyte invasion and induction of gametocytogenesis (Kaushal et al. Reference Kaushal, Carter, Miller and Krishna1980; McColm et al. Reference McColm, Hommel and Trigg1980; Brockelman, Reference Brockelman1982; Rangachari et al. Reference Rangachari, Dluzewski, Wilson and Gratzer1986; Trager and Gill, Reference Trager and Gill1989; Syin et al. Reference Syin, Parzy, Traincard, Boccaccio, Joshi, Lin, Yang, Assemat, Doerig and Langsley2001; Wurtz et al. Reference Wurtz, Desplans and Parzy2009a). More recently, several studies have implicated PfPKAc in the following processes: (i) activation of a Ca2+ influx (Beraldo et al. Reference Beraldo, Almeida, da Silva and Garcia2005; Wurtz et al. Reference Wurtz, Desplans and Parzy2009a), (ii) regulation of anion transport through the erythrocyte membrane (Merckx et al. Reference Merckx, Nivez, Bouyer, Alano, Langsley, Deitsch, Thomas, Doerig and Egee2008b, Reference Merckx, Bouyer, Thomas, Langsley and Egee2009), (iii) regulation of apical exocytosis and motility of sporozoites (Ono et al. Reference Ono, Cabrita-Santos, Leitao, Bettiol, Purcell, Diaz-Pulido, Andrews, Tadakuma, Bhanot, Mota and Rodriguez2008; Kebaier and Vanderberg, Reference Kebaier and Vanderberg2009) and (iv) mitochondrial protein traffic (Wurtz et al. Reference Wurtz, Desplans and Parzy2009a). Thus, PfPKA seems to be a key regulator of P. falciparum development and consequently represents an attractive target for the development of anti-malarial compounds.
PfPKA has a key role in the P. falciparum asexual life cycle
The catalytic and regulatory subunits of PfPKA are expressed weakly during the ring and trophozoite stages compared to the schizont stage, and pfpkac mRNA levels are lower in gametocytes and gametes (Syin et al. Reference Syin, Parzy, Traincard, Boccaccio, Joshi, Lin, Yang, Assemat, Doerig and Langsley2001; Bozdech et al. Reference Bozdech, Llina, Pulliam, Wong, Zhu and DeRisi2003; Ward et al. Reference Ward, Equinet, Packer and Doerig2004; Wurtz et al. Reference Wurtz, Desplans and Parzy2009a). Indeed, PfPKA seems to be essential for parasite growth and survival, as already described in previous studies: (a) H89, which inhibits PfPKAc activity in vitro, leads to parasite growth arrest and morphological alteration (Syin et al. Reference Syin, Parzy, Traincard, Boccaccio, Joshi, Lin, Yang, Assemat, Doerig and Langsley2001); (b) the parasite cell cycle is altered after treatment with an activator of PfPKAc (6-Bz-cAMP) (Beraldo et al. Reference Beraldo, Almeida, da Silva and Garcia2005); (c) transgenic parasites that overexpress PfPKAr have growth defects that can be restored by increasing the levels of intracellular cAMP (Merckx et al. Reference Merckx, Nivez, Bouyer, Alano, Langsley, Deitsch, Thomas, Doerig and Egee2008b) and (d) down-regulation of pfpkac mRNA using gene silencing leads to morphological changes in schizont stages and cell cycle arrest (Wurtz et al. Reference Wurtz, Desplans and Parzy2009a). Down-regulation of pfpkac mRNA using gene silencing is also associated with a compensatory decrease in pfpkar mRNA levels, suggesting a transcriptional self-regulation of the PfPKA signalling network. The parasites appear to have tightly controlled mechanisms for self-regulating PfPKA levels to maintain appropriate PKA signalling. This type of self-regulation has also been described in mammalian cells, where, for example, knocking down the regulatory subunit causes a subsequent decrease in levels of the catalytic subunit (Duncan et al. Reference Duncan, Moss and Williams2006). This phenomenon was already proposed for P. falciparum because over-expression of the regulatory subunit leads to an increase in pfpkac transcript levels (Merckx et al. Reference Merckx, Nivez, Bouyer, Alano, Langsley, Deitsch, Thomas, Doerig and Egee2008b). This PfPKA self-regulation mechanism might exist to counteract the adverse effects caused by changes in the expression levels of either PfPKAc or PfPKAr.
Despite the established importance of PfPKA during parasite growth, its substrates have not been clearly identified. However, several studies presented below have shown that PfPKA is involved in many signal transduction pathways.
Putative role for PfPKA in the induction of gametocytogenesis
Several previous reports have shown that cAMP levels appear to be important for the induction of gametocytogenesis (without the direct involvement of PfPKAc). Kaushal et al. (1980) have shown that static cultures of ring stages develop into gametocytes following the addition of 1 mm cAMP. Treatment of P. falciparum cultures with cAMP agonists or with phosphodiesterase inhibitors such as caffeine and 8-Br-cAMP results in an increase in gametocyte induction (Brockelman, Reference Brockelman1982; Trager and Gill, Reference Trager and Gill1989). Moreover, AC activity and cAMP levels have been correlated with the parasite's ability to produce gametocytes (Read and Mikkelsen, Reference Read and Mikkelsen1991a). More recently, Dyer and Day (Reference Dyer and Day2000) have shown that the addition of cholera toxin, which prevents AC inactivation, causes an increase in conversion to sexual development. However, to date, no other studies have been conducted to evaluate whether or not PfPKA is involved in the induction of gametocytogenesis.
PfPKA is implicated in sporozoite motility and hepatocyte invasion
Recently, the cAMP pathway was shown to regulate sporozoite motility and hepatic cell invasion by P. falciparum sporozoites (Ono et al. Reference Ono, Cabrita-Santos, Leitao, Bettiol, Purcell, Diaz-Pulido, Andrews, Tadakuma, Bhanot, Mota and Rodriguez2008; Kebaier and Vanderberg, Reference Kebaier and Vanderberg2009). Sporozoites are deposited in the host's skin by infected mosquitoes and must penetrate cell barriers in the skin and liver sinusoid to reach their target cell, the hepatocyte; once there, they enter in a vacuole and begin the next stage of their life cycle (Fig. 5) (Mota et al. Reference Mota, Hafalla and Rodriguez2002; Mota and Rodriguez, Reference Mota and Rodriguez2002; Ejigiri and Sinnis, Reference Ejigiri and Sinnis2009).
Schematic model of signalling events including PfPKAc during the Plasmodium falciparum life cycle. The P. falciparum life cycle requires 2 different hosts, an Anopheles mosquito and a human. When an infected mosquito takes a bloodmeal, it injects sporozoites that rapidly move to the liver through the bloodstream. They then progress through the liver cells and ultimately invade a single hepatocyte, where they develop into thousands of merozoites. The cAMP/PfPKAc pathway has been shown to regulate sporozoite motility and the apical exocytosis steps necessary for the invasion of hepatic cells. Next, the hepatocyte bursts and releases the merozoites into the bloodstream, where they invade RBCs. Asexual replication progresses through a series of stages (ring, trophozoite and schizont) that ends with the rupture of the RBC, releasing merozoites that can then reinvade new RBCs. During the asexual life cycle, PfPKAc has been shown to play a role in schizont maturation, merozoite release and in the reinvasion of new RBCs. More specifically, PfPKAc might have different functions in signal transduction events, as follows. (1) A highly complex interplay exists between the cAMP/PfPKAc and Ca2+ signalling pathways. First, activation of phospholipase C (PLC) generates inositol 1,4,5-triphosphate (IP3), which binds to its receptor (IP3R) located on the membrane of the endoplasmic reticulum (ER). This leads to calcium release into the cytoplasm that in turns activates AC and induces cAMP synthesis. cAMP binds to the PKA regulatory subunit and leads to the release and activation of the catalytic subunit. The increased calcium concentration initiates an amplification loop via cAMP and PKA, which in turns leads to a further increase in cytoplasmic calcium either by stimulating PLC or IP3R directly, or by calcium entry from outside of the cell. (2) cAMP-pathway components are involved in the regulation of anion conductance at the erythrocyte membrane. Despite lacking a Plasmodium export element/host targeting motif (PEXEL/HT), PfPKAc can be exported to the host cytosol, where it directly phosphorylates anion channels (AN) and/or eventually participates in NPP (new permeation pathway) formation. Alternatively, PfPKAc could either be exported to the erythrocyte cytosol where it phosphorylates proteins of human or parasite origin, or could phosphorylate an unidentified parasite substrate that is then exported to the host cytosol. Furthermore, if human PKAc is activated by parasite cAMP, it could also contribute to the induction of anion conductance. (3) PfPKAc may regulate some mitochondrial protein traffic. (4) PfPKAc certainly has many other cellular targets that are still unknown. In each erythrocyte cycle, some merozoites arrest their cell cycle and develop into sexual forms (gametocytes). A role for PfPKAc in gametocytogenesis induction has been proposed. The cycle is completed when a mosquito takes its bloodmeal and ingests male (♂) and female (♀) gametocytes. Question marks represent the suggested role of PfPKAc during the various events cited above. Maurer's clefts (MC), vesicles (V), tubovesicular network (TVN), red blood cell membrane (RBCM), parasitophorous vacuolar membrane (PVM), parasite plasma membrane (PPM), dense granule (DG), apicoplast (A), food vacuole (FV), cytostome (C), golgi (go), mitochondria (m), channel (C).

Cell invasion and gliding motility of sporozoites are active processes that are tightly associated with exocytosis of apical organelles in different Apicomplexans (Carruthers et al. Reference Carruthers, Giddings and Sibley1999). Sporozoites possess 2 types of secretory apical organelles: micronemes and rhoptries. Migration through cells activates the exocytosis of sporozoite apical organelles (Mota et al. Reference Mota, Hafalla and Rodriguez2002), which results in the release of parasite molecules that are essential for invasion. Two Plasmodium sporozoite microneme proteins that have been shown to be released during motility and invasion are circumsporozoite protein (CSP) and thrombospondin-related anonymous protein (TRAP) (Khan et al. Reference Khan, Ng and Vanderberg1992; Spaccapelo et al. Reference Spaccapelo, Naitza, Robson and Crisanti1997). Ono et al. (Reference Ono, Cabrita-Santos, Leitao, Bettiol, Purcell, Diaz-Pulido, Andrews, Tadakuma, Bhanot, Mota and Rodriguez2008) have shown that apical exocytosis is induced by increases in cAMP levels in the sporozoites of rodent and human Plasmodium species. Increasing the cytosolic cAMP level in Plasmodium sporozoites with the addition of the cell-permeable compounds 8-Br-cAMP or forskolin induces apical exocytosis in vitro, as measured by an increase in the accumulation of extracellular TRAP at the apical end of sporozoites. Moreover, incubation of sporozoites with AC inhibitors (MDL12330A, SQ22536) prevented sporozoite exocytosis. Thus, it is suggested that the synthesis of cAMP by AC increases sporozoite exocytosis. Indeed, treatment of P. yoelii sporozoites with 8Br-cAMP or forskolin was shown to decrease their ability to migrate through monolayers of the hepatoma cell line Hepa 1–6 and increase their ability to invade. The major downstream effector of cAMP is PfPKA, and direct inhibition of its activity by H89 or Rp-cAMP was also able to significantly reduce sporozoite exocytosis, suggesting that this process is mediated by PfPKA activation (Ono et al. Reference Ono, Cabrita-Santos, Leitao, Bettiol, Purcell, Diaz-Pulido, Andrews, Tadakuma, Bhanot, Mota and Rodriguez2008). Pre-treatment of sporozoites with H89 followed by induction of cAMP synthesis by 8-Br-cAMP completely inhibited exocytosis, suggesting that PKA activation occurs after cAMP generation. In the P. falciparum genome, 2 genes coding for AC have been identified (ACα and ACβ) (Baker and Kelly, Reference Baker and Kelly2004) and their expression demonstrated in sporozoites (Le Roch et al. Reference Le Roch, Zhou, Blair, Grainger, Moch, Haynes, De laVega, Holder, Batalov, Carucci and Winzeler2003). Deletion of P. berghei ACα does not alter parasite growth during blood stages or in the mosquito, but mutant sporozoites are not able to expose the adhesive proteins and their infectivity is reduced by 50% (Ono et al. Reference Ono, Cabrita-Santos, Leitao, Bettiol, Purcell, Diaz-Pulido, Andrews, Tadakuma, Bhanot, Mota and Rodriguez2008). Re-introduction of ACα in deficient parasites resulted in a complete recovery of exocytosis and infection. These data reveal the importance of cAMP and PfPKA in sporozoite apical-regulated exocytosis, which is involved in hepatocyte infection by sporozoites.
Kebaier and Vanderberg (Reference Kebaier and Vanderberg2009) subsequently focused on motility rather than invasion by using albumin, which triggers motility in Plasmodium sporozoites, and evaluated the link between sporozoite exposure to albumin and intracellular signalling pathways, especially cAMP and calcium networks. First, they have shown that parasite intracellular calcium is necessary for sporozoite motility. Use of a calcium chelator (BAPTA-AM) inhibits sporozoite motility, and these effects are reversed by the addition of exogenous calcium (calcium ionophore A23187). Moreover, they have demonstrated that suppression of cAMP synthesis by an AC inhibitor (SQ22536) also leads to a decrease in sporozoite motility. The same results were obtained when the sporozoites were treated with PKA inhibitor H89 or Rottlerin (a non-specific kinase inhibitor). Thus, elevating the concentration of cAMP (by addition of forskolin, IBMX or cAMP analogues) allows for sporozoite motility without the addition of albumin in the medium. This study revealed that calcium and cAMP/PKA pathways act together to promote sporozoite motility.
A highly complex relationship between cAMP/PfPKA and calcium pathways exists in the P. falciparum asexual life cycle
Beraldo et al. (Reference Beraldo, Almeida, da Silva and Garcia2005) studied in detail the involvement of cAMP and its target PfPKAc in calcium signalling mechanisms during P. falciparum intraerythrocytic development. They demonstrated that melatonin, by activating specific receptors coupled to phospholipase C activation, causes the release of calcium from P. falciparum intracellular compartments in vitro (Hotta et al. Reference Hotta, Gazarini, Beraldo, Varotti, Lopes, Markus, Pozzan and Garcia2000). Subsequently, they observed that melatonin increases cAMP levels and PfPKAc activity, suggesting an important role for calcium in the control of cAMP production. When iRBCs were treated with 6-Bz-cAMP or IBMX (PfPKAc activators), there was a change in the parasite cell cycle and an increase in the schizont population, similar to that observed when parasites were treated with melatonin. The effects of melatonin were abolished by adding PfPKAc inhibitors (PKI, H89, Rp-cAMP). These data suggest that cAMP and PKA are key modulators of the P. falciparum cell cycle (Fig. 5). Inhibition of phospholipase C by U73122 blocks the melatonin-induced cAMP increase. On the other hand, the addition of exogenous calcium leads to an augmentation of cAMP levels. These data suggest that the increase in cAMP levels is directly caused by an increase in calcium concentration caused by melatonin, rather than by a coupling of the melatonin receptors to AC (Beraldo et al. Reference Beraldo, Almeida, da Silva and Garcia2005). However, the interplay between cAMP and calcium is not limited to the calcium-dependent activation of cAMP production. In fact, PKA activator 6BZcAMP is able to induce calcium level increases in the parasite, either by mobilizing calcium from intracellular compartments or by stimulating calcium entry from the medium. Beraldo et al. (Reference Beraldo, Almeida, da Silva and Garcia2005) concluded that the modulation of the P. falciparum cell cycle by the host hormone melatonin is mediated by 2 second messengers acting together. (1) Melatonin is directly coupled to a classical calcium signalling pathway via phospholipase C, which cleaves phosphatidylinositol 4,5-bisphosphate into inositol 1,4,5-triphosphate (IP3). IP3 then diffuses through the cytosol to bind to IP3 receptors on calcium channels in the endoplasmic reticulum, which causes an increase in cytoplasmic calcium concentration. (2) The elevation of calcium concentration initiates an amplification cycle via cAMP and PKA, which in turn leads to an increase in cytoplasmic calcium either by calcium release from the endoplasmic reticulum or by stimulating calcium entry from the outside. Thus, there is a highly complex relationship between the calcium and cAMP signalling networks in Plasmodium. These data are consistent with another study showing that gene silencing of PfPKAc leads to a down-regulation of members of the calcium/calmodulin pathway, again suggesting an interplay between the cAMP and calcium networks (Wurtz et al. Reference Wurtz, Desplans and Parzy2009a).
PfPKA plays a key role in anion transport across the erythrocyte membrane during the P. falciparum asexual life cycle
While replicating in red blood cells (RBCs), P. falciparum is able to modify the host cell by increasing its permeability to facilitate nutrient uptake and to evacuate potentially dangerous metabolites for the cell (Kirk, Reference Kirk2001). The parasites can alter permeability of the erythrocyte membrane either by over-expressing existing carriers or by creating new permeation pathways (NPP). Egee et al. (Reference Egee, Lapaix, Decherf, Staines, Ellory, Doerig and Thomas2002) found that the anion channels of uninfected erythrocytes could be activated by the addition of bovine PKA and ATP, producing a membrane current similar to that observed in P. falciparum-infected red blood cells (iRBCs) and suggesting that the mechanism of regulation used by the parasite may involve phosphorylation steps (Egee et al. Reference Egee, Lapaix, Decherf, Staines, Ellory, Doerig and Thomas2002). Additionally, Merckx et al. Reference Merckx, Nivez, Bouyer, Alano, Langsley, Deitsch, Thomas, Doerig and Egee(2008b) recently reported that the addition of exogenous PfPKAr protein to P. falciparum iRBCs leads to a down-regulation of whole-cell membrane conductance, probably regulated by cAMP. Thus, exogenous PfPKAr seems to interfere with the parasite-dependent activation of iRBC membrane conductance. Moreover, these authors generated a P. falciparum strain over-expressing PfPKAr and observed that the transgenic parasite produces a clearly reduced membrane current, similar to that observed after the addition of exogenous PfPKAr. They also tested whether the over-expression of PfPKAr interferes with NPP activity by using semi-quantitative haemolysis experiments with sorbitol as permeating substrate. The transgenic parasites displayed decreased membrane permeability to sorbitol since the lysis duration was significantly increased compared with control cultures. Thus, the delay observed in haemolysis for the parasites over-expressing PfPKAr suggests that some NPP activity is under the dependence of phosphorylation via cAMP dependent protein kinases. In addition, several mechanisms have been proposed regarding the function of PfPKAc during anion conductance regulation (Merckx et al. Reference Merckx, Bouyer, Thomas, Langsley and Egee2009). It seems that PfPKAc regulates anionic conductance, either via direct phosphorylation of the channels or indirectly, through phosphorylation of accessory or associated proteins that can be of human or parasite origin (Fig. 5).
Putative role for PfPKA in erythrocyte invasion by merozoites
Several studies have demonstrated roles for the cAMP/PKA and calcium/calmodulin pathways in P. falciparum erythrocyte invasion by merozoites (Rangachari et al. Reference Rangachari, Dluzewski, Wilson and Gratzer1986; Green et al. Reference Green, Rees-Channer, Howell, Martin, Knuepfer, Taylor, Grainger and Holder2008; Wurtz et al. Reference Wurtz, Desplans and Parzy2009a). The expression of 6 reticulocyte-binding-like (RBL) homologue genes was found to be down-regulated in response to pfpkac mRNA inhibition (Wurtz et al. Reference Wurtz, Desplans and Parzy2009a). These genes belong to the invasion/motility pathway and seem to be important for P. falciparum invasion of human erythrocytes (Tham et al. Reference Tham, Wilson, Reiling, Chen, Beeson and Cowman2009). To date, only indirect data have demonstrated the potential role of PfPKAc in this specific pathway (McColm et al. Reference McColm, Hommel and Trigg1980; Rangachari et al. Reference Rangachari, Dluzewski, Wilson and Gratzer1986; Syin et al. Reference Syin, Parzy, Traincard, Boccaccio, Joshi, Lin, Yang, Assemat, Doerig and Langsley2001). While PfPKAc seems to be involved via the RBL genes in RBC invasion by the parasite, the precise roles of the cAMP/PKA and calcium/calmodulin pathways in this process still need to be elucidated.
Putative role for PfPKA in the regulation of mitochondrial protein traffic
Another unexpected pathway that could involve the cAMP network concerns genes related to mitochondrial functions (Wurtz et al. Reference Wurtz, Desplans and Parzy2009a). Many nuclear genes with mitochondrial signal sequences were found to be induced when pfpkac expression was inhibited (Wurtz et al. Reference Wurtz, Desplans and Parzy2009a). It is well known that parasite mitochondrial activity requires the import of many proteins (van Dooren et al. Reference van Dooren, Stimmler and McFadden2006; Torrentino-Madamet et al. Reference Torrentino-Madamet, Desplans, Travaille, James and Parzy2009). PfPKAc may thus regulate part of the mitochondrial protein traffic, as has already been described for mammalian cells (De Rasmo et al. Reference De Rasmo, Panelli, Sardanelli and Papa2008).
PROTEIN KINASE CELLULAR SIGNALLING AS A POTENTIAL TARGET FOR THERAPEUTIC INTERVENTION
ATP binding, substrate binding and/or kinase activity are all potential targets for inhibition by drugs designed to block protein kinases. In 2008, 10 protein kinase inhibitors had been approved for clinic use, and there are many more in clinical trials (Johnson, Reference Johnson2009). P. falciparum contains members of most of the established protein kinase families (Ward et al. Reference Ward, Equinet, Packer and Doerig2004). However, the differences between the host and parasite phosphosignalling pathways suggest that specific inhibition of the latter can be accomplished (Leroy and Doerig, Reference Leroy and Doerig2008). This notion was confirmed by 2 structural studies demonstrating exploitable divergences between host and parasite protein kinases (Holton et al. Reference Holton, Merckx, Burgess, Doerig, Noble and Endicott2003; Merckx et al. Reference Merckx, Echalier, Langford, Sicard, Langsley, Joore, Doerig, Noble and Endicott2008a). In the case of PfPKA, we have shown here that it presents interesting differences in terms of sequence and structure compared to human PKA. These differences involve ATP anchoring, PfPKAc substrate recognition and phosphorylation, sensitivity of PfPKAc to kinase inhibitors and the D/D domain and inhibitory sequence of PfPKAr. Thus, specifically targeting these domains together or separately could be an effective strategy for inhibiting the parasite enzyme without interfering with the equivalent host protein.
Targeting the kinase activity directly
Most of the protein kinase inhibitors currently in clinical trials for cancer therapy are small molecules that compete for the ATP-binding site. A major success in this category of inhibitors is the tyrosine kinase inhibitor imatinib (Gleevec®, Novartis), a potent inhibitor of the constitutively active BCR-ABL fusion protein that is used for the treatment of leukaemia and gastrointestinal stromal tumours (Druker, Reference Druker2002; Tibes et al. Reference Tibes, Trent and Kurzrock2005). This has been followed by other small molecules such as the epidermal growth factor receptor inhibitors erlotinib (Tarceva™ Genentech) and gefitinib (Iressa™ AstraZeneca), both of which received approval for the treatment of non-small cell lung carcinoma (Modjtahedi and Essapen, Reference Modjtahedi and Essapen2009). As mentioned above, the ATP-binding site of PfPKAc presents some differences when compared to that of human PKAc, suggesting that the design of molecules specifically targeting the parasite domain may be feasible.
Another strategy to inhibit the activity of a protein kinase is to prevent the translation of its transcripts. This can be achieved using ribozymes, which are modified RNA molecules that can cut other RNA. Ribozymes consist of a central catalytic domain with RNA-degrading activity, flanked by RNA sequences that are complementary to the target mRNA. RPI.4610 (Angiozyme) was the first synthesized ribozyme to be studied in human trials. It is designed to prevent the process of angiogenesis by cleaving the mRNA encoding the VEGF1 receptor (Perabo and Muller, Reference Perabo and Muller2007). LErafAON, an antisense oligonucleotide targeting the serine/threonine kinase c-Raf that has been implicated in many cancers, has been tested in phase I clinical trials (Wellbrock et al. Reference Wellbrock, Karasarides and Marais2004; Zhang et al. Reference Zhang, Newsome, Mewani, Pei, Gokhale and Kasid2009). This type of approach could be used to inhibit the expression of PfPKAc by designing ribozymes that specifically target the PfPKAc mRNA without altering human PKAc expression.
Targeting partners of kinases or effectors of the pathway
Rather than directly inhibiting the active enzyme, other strategies can be considered that target either the partners or the upstream and/or downstream effectors of the pathway. One possibility is to target the regulatory subunit of PKA, especially for cancer therapy, as its protein and mRNA levels have been found to be upregulated in a series of transformed cell lines and human neoplasms (Bradbury et al. Reference Bradbury, Carter, Miller, Cho-Chung and Clair1994; Miller, Reference Miller2002). GEM®231 (HYB165, Hybridon) is an 18-mer antisense oligonucleotide targeted against human PKA RIα. Used alone or in combination with other agents, GEM®231 has demonstrated anti-tumour activity in a variety of in vitro cancer cells and in vivo human tumour xenograft models (Tortora and Ciardiello, Reference Tortora and Ciardiello2002; Wang et al. Reference Wang, Hang, Shi, Li, Yu, Kandimalla, Agrawal and Zhang2002). We can imagine designing an antisense oligonucleotide against PfPKAr targeting the C-terminal end of the sequence, as we have demonstrated above a significant difference between PfPKAr and human PKAr in this region.
The AKAPs introduce another level of complexity to PKA signalling and have emerged as key regulators of PKA function. To date, these partners have not yet been well studied but appear as interesting therapeutic targets, particularly in the treatment of severe cardiac pathologies and cancers (Diviani, Reference Diviani2008; Naviglio et al. Reference Naviglio, Caraglia, Abbruzzese, Chiosi, Di Gesto, Marra, Romano, Sorrentino, Sorvillo, Spina and Illiano2009). In the case of P. falciparum, the hypothetical AKAP identified by orthology presents only 22% identity with human AKAP18. Thus, we propose specifically targeting either the parasite AKAP or the interaction between AKAP and PfPKAr because, as noted above, the mechanism of interaction between these two partners seems to be different from that of their human homologues.
Interfering with the function of protein kinases can be achieved with substrate-mimicking molecules that compete with the original substrate. By occupying the natural binding site of the substrate, these molecules end the signal transduction events that help maintain the pathogenic state of the cell. The substrate mimic Thymectacin™ (NB1011), which targets thymidylate synthase, an enzyme overexpressed in tumours, has entered clinical trials (Congiatu et al. Reference Congiatu, McGuigan, Jiang, Davies and Mason2005). Therefore, this strategy of inhibiting enzymatic activity has potential clinical applications. However, substrate competitive inhibitors targeting protein kinases have not yet entered clinical trials, and the substrates of PfPKAc have not yet been clearly defined, hampering the development of such molecules.
A different way to restrain protein kinase activity is to block the upstream activation of the pathway using small molecules or antibodies that prevent receptor-mediated signalling. In the case of the PKA signalling pathway, several upstream partners can be targeted to alter kinase function, including G-protein coupled receptors, adenylate cyclase and phosphodiesterase (Wise et al. Reference Wise, Gearing and Rees2002; Zhang et al. Reference Zhang, Ibrahim, Gillette and Bollag2005; Pavan et al. Reference Pavan, Biondi and Dalpiaz2009). In 2000, 26 of the top 100 pharmaceutical products were compounds that target GPCRs, including salmeterol (asthma), sumatriptan (migraine), ibuprofen (inflammation, pain), rimonabant (obesity), haloperidol (schizophrenia), cabergoline (Parkinson's disease) and many more (Wise et al. Reference Wise, Gearing and Rees2002). Phosphodiesterases play crucial roles in cell signalling and have therefore been the target of clinical drug development for indications ranging from anti-inflammation to memory enhancement. Many drugs targeting such proteins have been developed, including theophylline (asthma), anagrelide (thrombocytosis), milrinone (cardiac failure) and dipyridamole (inhibitor of platelet aggregation) (Wise et al. Reference Wise, Gearing and Rees2002; Zhang et al. Reference Zhang, Ibrahim, Gillette and Bollag2005; Denault et al. Reference Denault, Lamarche, Couture, Haddad, Lambert, Tardif and Perrault2006; Chakrabarti and Freedman, Reference Chakrabarti and Freedman2008; Emadi and Spivak, Reference Emadi and Spivak2009). Although many drugs target the cAMP signalling pathway through G-protein coupled receptors or phosphodiesterases, adenylate cyclases have not yet been considered as drug targets. However, the generation of knockout and transgenic animals has revealed that these proteins have crucial roles in numerous biological processes (Pierre et al. Reference Pierre, Eschenhagen, Geisslinger and Scholich2009). Mammalian adenylate cyclases are currently under investigation as potential drug targets, with some compounds already being used in clinics. For example, corlforsin has been approved in Japan for the treatment of heart failure (Ogata et al. Reference Ogata, Segawa and Minami2007). These PfPKAc partners could be considered as potential drug targets; however, more work is needed on these genes, which have not yet been well characterized.
Another approach to inhibiting the PKA pathway is the use of cAMP analogues. Between 1960 and 1980, numerous analogues of cAMP were synthesized and screened for their therapeutic potential, especially against diabetes, asthma and cardiovascular diseases. A good illustration is 8-Cl-cAMP which inhibits cancer cell growth through both anti-proliferation and pro-apoptotic mechanisms (Cho-Chung and Nesterova, Reference Cho-Chung and Nesterova2005). This molecule has completed several phase I clinical studies and recently entered phase II clinical trials as an anticancer agent (Tortora and Ciardiello, Reference Tortora and Ciardiello2002). However, the strategy of using cAMP analogues does not seem feasible in the case of P. falciparum because the interactions between cAMP and PfPKAr appear similar to those in humans; therefore, these compounds would not specifically target the parasite. In conclusion, PfPKA and the P. falciparum cAMP pathways appear to be relevant biological targets for the therapy and management of malaria.
CONCLUSIONS AND PERSPECTIVES
In spite of its established importance during parasite growth and the different pathways that are associated with it, the substrates of PfPKA have not yet been clearly identified. Merckx et al. (Reference Merckx, Bouyer, Thomas, Langsley and Egee2009) identified several PfPKAc substrates in human RBCs and in the P. falciparum proteome by using an in silico search for phosphorylation sites using PkaPS (Prediction of protein kinase A Phosphorylation Sites, http://mendel.imp.ac.at/sat/pkaPS/pkaPS.html) (Neuberger et al. Reference Neuberger, Schneider and Eisenhaber2007). As the recombinant PfPKAc and PfPKAr proteins are available, different strategies could be employed to identify both the upstream targets and specific inhibitors of this enzyme. First, recombinant PfPKAc could be used to test the protein's capacity to phosphorylate potential parasite/human substrates using the KESTREL (kinase substrate tracking and elucidation) approach (Cohen and Knebel, Reference Cohen and Knebel2006; Peng et al. Reference Peng, Knebel, Morrice, Li, Barringer, Li, Jakes, Werneburg and Wang2007; Philip and Haystead, Reference Philip and Haystead2007). This strategy has been applied successfully to P. falciparum to identify the substrates of serine / threonine kinase PfPK9 (Philip and Haystead, Reference Philip and Haystead2007). To avoid the use of radioactive molecules, detection of phosphorylated proteins can be achieved using specific fluorescent staining allowing direct, in-gel detection of phosphate groups attached to tyrosine, serine or threonine residues (e.g., ProQ® Diamond, Invitrogen) (Schulenberg et al. Reference Schulenberg, Goodman, Aggeler, Capaldi and Patton2004; Orsatti et al. Reference Orsatti, Forte, Tomei, Caterino, Pessi and Talamo2009). In addition, the use of protein kinase inhibitors, such as H89, on P. falciparum could reveal novel substrates, potential new pathway interconnections and inhibitor specificity by monitoring differences in protein levels and phosphorylation (Davis et al. Reference Davis, Hinerfeld, Joseph, Hui, Huang, Leszyk, Rutherford, Bethard and Tam2006).
Thus recombinant proteins obtained can also be used (i) to produce specific anti-PfPKAc and anti-PfPKAr antibodies to determine the cellular locations of PfPKAc, PfPKAr and their partners (Murtaugh et al. Reference Murtaugh, Steiner and Davies1982; Ray et al. Reference Ray, Chen and Ray2001), and (ii) to perform high-throughput screening of PfPKAc inhibitors and interaction studies with PfPKAr (Merckx et al. Reference Merckx, Nivez, Bouyer, Alano, Langsley, Deitsch, Thomas, Doerig and Egee2008b; Blackwell et al. Reference Blackwell, Birkos, Hallam, Van De Carr, Arroway, Suto and Janzen2009). Clearly, the identification of the upstream signals/molecular events that regulate PfPKAc activity and their downstream targets will be crucial for a more precise understanding of their cellular function and should also provide new targets for drug design.
ACKNOWLEDGEMENTS
The authors would like to thank Dr Boris Pastorino, Dr Lionel Bertaux, Stéphane Pelleau and Dr Sébastien Briolant for critical readings of the manuscript, and Professor Susan Taylor, Dr Alexander Kornev and Professor Kottayil Varughese for their help with the B. taurus PKAr structure. The opinions and assertions contained herein are those of the authors and are not to be construed as official or reflecting the views of the French Armed Forces Medical Service or the French Army at large. All authors declare that they have no conflict of interest. This work was supported by the French Armed Forces Medical Service and the French ‘Délégation Générale pour l'Armement’ (grant number 06co008).



