Implications
Feed additives, such as antibiotics, have proven to be effective by improving nutrient utilization, leading to improved feed conversion and better growth rate (Parker and Armstro, Reference Parker and Armstro1987; Gartner and O’Rourke, Reference Gartner and O’Rourke1997). However, there is increasing public concern about the use of feed antibiotics in livestock production due to the possible development of drug resistance in human pathogenic bacteria (Solomons, Reference Solomons1978). Thus, antibiotics are banned within the EU (Casewell et al., Reference Casewell, Friis, Marco, McMullin and Phillips2003). Accordingly, the scientific community and animal feed industry have been actively searching for alternatives to feed antibiotics and growth promoters to manipulate rumen fermentation and to improve feed efficiency. Malic acid (MA) is a four-carbon dicarboxylic acid that is an intermediate in the succinate–propionate pathway of ruminal bacteria. Although in vitro studies have shown positive effects of MA on ruminal fermentation, limited in vivo studies are available to evaluate the effects of MA on rumen fermentation and feed efficiency. Therefore, the aim of this work was to study the effects of MA supplementation on ruminal pH and fermentation, urinary excretion of purine derivatives (PDs) and nutrient digestibility in beef cattle.
Introduction
Feed additives, such as antibiotics, have proven to be effective by improving nutrient utilization, leading to improved feed conversion and better growth rate (Parker and Armstro, Reference Parker and Armstro1987; Gartner and O’Rourke, Reference Gartner and O’Rourke1997). However, there is increasing public concern about the use of feed antibiotics in livestock production due to the possible development of drug resistance in human pathogenic bacteria (Solomons, Reference Solomons1978; Casewell et al., Reference Casewell, Friis, Marco, McMullin and Phillips2003). Accordingly, the scientific community and animal feed industry have been actively searching for alternatives to feed antibiotics and growth promoters to manipulate rumen fermentation and to improve feed efficiency.
MA is a four-carbon dicarboxylic acid that is an intermediate in the succinate–propionate pathway of ruminal bacteria (Castillo et al., Reference Castillo, Beneditio, Méndez, Pereira, López-Alonso, Miranda and Hernández2004). In vitro, MA increased concentrations of propionate and total volatile fatty acid (VFA) (Martin and Streeter, Reference Martin and Streeter1995; Martin et al., Reference Martin, Streeter, Nisbet, Hill and Williams1999; Carro and Ranilla, Reference Carro and Ranilla2003), decreased methane production (Carro and Ranilla, Reference Carro and Ranilla2003) and lactate concentration (Nisbet and Martin, Reference Nisbet and Martin1991; Carro and Ranilla, Reference Carro and Ranilla2003), and increased the digestibility of dry matter (DM), organic matter (OM), neutral detergent fiber (NDF) and hemicellulose (Carro et al., Reference Carro, López, Valdés and Overjero1999). However, the results from animal studies are inconclusive. The addition of MA to diets increased the average daily gain (ADG) and feed efficiency in calves (Sanson and Stallcup, Reference Sanson and Stallcup1984) and feedlot steers (Streeter et al., Reference Streeter, Nisbet, Martin and Williams1994). MA supplementation increased digestibilities of acid detergent fiber (ADF) and NDF (Sniffen et al., Reference Sniffen, Ballard, Carter, Cotanch, Danna, Grant, Mandebvu, Suekawa and Martin2006). In other trials, MA increased ruminal propionate (Gómez et al., Reference Gómez, Tejido and Carro2005) and butyrate production (Gómez et al., Reference Gómez, Tejido and Carro2005; Carro et al., Reference Carro, Ranilla, Giráldez and Mantecón2006), and decreased the ratio of methane to VFA (Gómez et al., Reference Gómez, Tejido and Carro2005). In contrast, there were no effects of MA on ruminal pH (Gómez et al., Reference Gómez, Tejido and Carro2005; Sniffen et al., Reference Sniffen, Ballard, Carter, Cotanch, Danna, Grant, Mandebvu, Suekawa and Martin2006), ruminal total VFA, propionate, butyrate and isobutyrate production (Sniffen et al., Reference Sniffen, Ballard, Carter, Cotanch, Danna, Grant, Mandebvu, Suekawa and Martin2006), ruminal digestion and rumen microbial efficiency (Montaño et al., Reference Montaño, Chai, Zinn-Ware and Zinn1999), diet digestibility and N retention (Kung et al., Reference Kung, Huber, Krummrey, Allison and Cook1982). In field trials, MA supplementation did not affect feed intake, total tract digestibility or lamb growth performance (Carro et al., Reference Carro, Ranilla, Giráldez and Mantecón2006).
These contrasting results could be due to differences in the composition of the diet and/or to the dose of MA. Across the reported studies, there was a wide range in supplementation level of MA. In addition, Castillo et al. (Reference Castillo, Beneditio, Méndez, Pereira, López-Alonso, Miranda and Hernández2004) suggested that dietary factors, such as forage to concentrate ratio and forage type, are important in determining responses to MA supplementation because the content of MA in the basal diet will vary. The MA content of forage varies with forage type (legumes > grasses), forage variety, maturity (immature > mature) and processing (fresh > hay or pelleting; Callaway et al., Reference Callaway, Martin, Wampler, Hill and Hill1997). However, information on the effects of dietary supplementation of MA on rumen fermentation, nutrient digestibility as well as the mode of action of MA in the digestive tract of ruminants is limited. Therefore, the aim of this work was to study the effects of MA supplementation on ruminal pH and fermentation, urinary excretion of PDs and nutrient digestibility in beef cattle.
Material and methods
Animals and experimental design
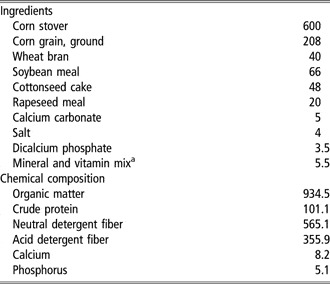
Eight ruminally cannulated Chinese Simmental steers averaging 3.0 years of age and 465 ± 13 kg of body weight (BW) were assigned to a replicated 4 × 4 Latin square design at random. The treatments were as follows: control (without MA), LMA (MA-low), MMA (MA-medium) and HMA (MA-high) with 0.0, 7.8, 15.6 and 23.4 g MA per kg DM, respectively. The food-grade MA supplement (99.8% of MA; Shandong Haiquan malic acid Co., Ltd, Xintai, China) was purchased commercially and was added in the concentrate portion when it was pelleted in the feed mill. The amount of MA fed was determined from previous work by Kung et al. (Reference Kung, Huber, Krummrey, Allison and Cook1982) who found that feeding 140 g of MA per day increased milk persistency in lactating cows and increased total VFA during early lactation. Diets consisted of corn stover and concentrate (60/40, DM basis) (Table 1). DM intake was approximately 9 kg per day, which was 90% of ad libitum intake including 5.4 kg corn stover and 3.6 kg concentrate. Experimental periods were 21 days with 11 days of adaptation and 10 days of sampling. Steers were housed in individual pens (3 × 3 m2) for the adaptation period. Steers were fed twice daily at 0700 and 1900 h and fresh water was available throughout the experimental period. Orts (residual fodder) were measured daily at 1600 h during the adaptation period, and the amount of feed offered was adjusted for a target of 5% orts. On day 8, steers were restricted to 90% of their average ad libitum intake determined during the prior 7 days in an attempt to assure no orts during the sampling periods. Samples of diets were collected once daily and then bulked across the week for DM determination, and then composited by period. The samples were dried in an oven at 55°C for 48 h, and ground to pass a 1-mm screen with a mill (FZ102; Shanghai Hong Ji Instrument Co., Ltd, Shanghai, China) for chemical analysis. The animals were weighed at the beginning and the end of each period. The experimental protocol was approved by the Animal Care and Use Committee of the Shanxi Agriculture University.
Ingredient and chemical composition of the basal diet (in g/kg dry matter)

aContained 42 ppm Co, 3500 ppm Cu, 20 000 ppm Fe, 12 000 ppm Mn, 12 000 ppm Zn, 1200 ppm I, 600 ppm Se, 3000 IU/g of vitamin A, 500 IU/g of vitamin D and 15 IU/g of vitamin E.
In situ ruminal degradability
Ruminal degradation kinetics of the corn stover and concentrate mix used in the present study was measured using the nylon bag technique (Ørskov et al., Reference Ørskov, DeB Hovell and Mould1980) on days 12 to 14 of the experimental period. The type of concentrate mix incubated in the rumen was the same as that in the diet. The corn stovers were ground to pass a 2.5-mm screen with a mill in order to determine the NDF contents conveniently after incubation. Approximately 3 g of corn stover and 4 g of concentrate were then weighed in 9 cm × 16 cm nylon bags made of monofilament Pecap polyester (Guangzhou Minyuan Business Co., Ltd, Guangdong, China) with a mean pore size of 47 ± 2 μm and heat-sealed. Individual bags were placed into the rumen through the ruminal fistula at 2 h after feeding (except the zero hour bags). The duplicated bags were suspended in the rumen of each steer for 0, 4, 8, 12, 24, 36, 48 and 72 h. An empty bag without sample for each incubation time was also incubated in the rumen as a blank bag (used to correct the foreign materials attached with nylon tissue). All bags were removed at the end of the incubation period and were manually rinsed in cold tap water until the effluent remained clear. The bags were subsequently dried at 65°C for 12 h and then at 100°C for 24 h. All bags were weighed to determine DM disappearance.
Kinetics of nutrient disappearance in situ in the rumen was estimated using the non-linear regression procedure of SAS (SAS, 1996). For each steer, period and type of feed, the following model was fitted to the percentage of nutrient disappearance (McDonald, Reference McDonald1981):

where a = soluble fraction, b = slowly degradable fraction, c = fractional degradation rate constant at which b is degraded, L = lag time (h) and t = time of incubation (h).
Effective degradability (ED) of feed was determined using ED = a + [bc/(c + k)], where k was the particulate passage rate out of the rumen and was 0.025 h−1 for corn stover and 0.058 h−1 for concentrate mix according to our measurements (Liu et al., Reference Liu, Wang, Huang, Dong, Yang and Wang2008) according to the procedure of Yang et al. (Reference Yang, Beauchemin, Koenig and Rode1997) using Cr-mordanted NDF and Yb acetate as forage and concentrate markers, respectively.
Ruminal pH and fermentation
Ruminal pH and fermentation characteristics were measured for two consecutive days, i.e. during days 19 and 20 of the period. At 0, 3, 6 and 9 h after the 0700 h feeding, 200 ml rumen fluid sample was taken manually with a small container from several sites within the rumen (dorsal and ventral sac) through the rumen cannula (the sample volume equal from different sites). Ruminal pH was immediately measured using an electric pH meter (Sartorius Basic pH Meter PB-20; Sartorius AG, Goettingen, Germany). The samples were then strained through four layers of cheesecloth. Five milliliters of filtrate was preserved by adding 1 ml of 250 g/l (w/v) meta-phosphoric acid to determine VFA and 5 ml of filtrate was preserved by adding 1 ml of 20 g/l (w/v) sulfate to determine ammonia nitrogen. The samples were subsequently stored frozen at −20°C until analyses.
Apparent digestibility in the total tract
Steers were dosed via ruminal cannula with 2 g of chromic oxide per day per steer in two equal proportions at 0700 and 1900 h beginning 7 days before sampling and continuing throughout the sampling period for use as a digestion marker. Fecal samples (approximately 200 g wet weight) were collected for each steer from the rectum three times daily at various times (3-h intervals) during five consecutive days and pooled by steer for each period. After being dried at 55°C for 48 h, the samples were ground in a feed mill to pass a 1-mm sieve for chemical analyses. DM excreted in feces was calculated by dividing chromium input (g chromium/day) by chromium concentration (g chromium/kg of DM) in the feces. Excretion of other nutrients in the feces was calculated by multiplying DM flow by their concentration in fecal DM.
Urine collection and PD measurements
Urine output (total urine excreted daily) was totally collected using urine collection aprons (Hobbs et al., Reference Hobbs, Hansard and Barrick1950; Liu et al., Reference Liu, Wang, Huang, Dong, Yang and Wang2008) from day 12 to 21 of the period. Urine was collected daily into containers by adding 10% sulfuric acid (sufficient to maintain pH < 3), weighed, mixed well and 1% daily aliquot was pooled over the 10-day period per animal. At the end of the collection period, 20 ml urine samples was diluted to 100 ml with distilled water, then divided into two subsamples and stored at −20°C for analysis of allantoin and uric acid. Urinary PD excreted (mmol/day) were estimated as the sum of uric acid and allantoin.
Chemical analyses
DM content of the ingredients (corn stover, concentrate mix) was determined by oven drying at 65°C for 24 h. Analytical DM content of oven-dried samples was determined by drying at 135°C for 3 h (AOAC, 1990; method 930.15). The OM content was calculated as the difference between DM and ash contents, with ash determined by combustion at 550°C for 5 h. The NDF and ADF contents were determined using the methods described by Van Soest et al. (Reference Van Soest, Robertson and Lewis1991) with heat-stable alpha amylase and sodium sulfite used in the NDF procedure and expressed inclusive of residual ash. Content of N in the samples was determined by the Kjeldahl method (AOAC, 1990; method 976.05). Ruminal VFA were separated and quantified by gas chromatography (GC102AF; Shanghai Specialties Ltd, Shanghai, China) using a 2-m (ϕ4-mm) fused PEG2000, Chromsob W AW DMCS column with 2-ethylbutyric acid as the internal standard. Ammonia N content of ruminal samples was determined using the method of AOAC (1990). Concentrations of lactic acid were determined (Sigma Procedure no. 826-UV; Sigma Chemical Co., St Louis, MO, USA) following the method of Montaño et al. (Reference Montaño, Chai, Zinn-Ware and Zinn1999). Allantoin and uric acid in urine was determined by an ultraviolet-visible spectrophotometer UV-2100 using the procedure of IAEA (1997).
Statistical analyses
Data were analyzed using the mixed-model procedure of SAS (Proc Mixed; SAS, 1996) to account for effects of square, period within square, animal within square and treatment. The treatment was considered a fixed effect; square, period within square and animal within square were considered random effects. Data for ruminal pH, VFA and ammonia N were summarized by sampling time and then analyzed using the same mixed model but with time included as a repeated measure using compound symmetry. Linear and quadratic orthogonal contrasts were tested using the CONTRAST statement of SAS with coefficients estimated based on the MA application rates. Effects of the factors were declared significant at P < 0.05 unless otherwise noted and trends were discussed at P < 0.10.
Results
Ruminal pH and fermentation
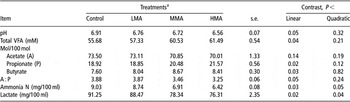
Ruminal pH, ammonia N, VFA profiles and lactate concentrations are shown in Table 2. Mean ruminal pH was linearly changed by altering the amount of MA supplementation but there was no quadratic effect observed with increase in MA supplementation. Total ruminal VFA concentration was higher for MA supplementation (59.78 mM) than for control (55.68 mM). However, differences in total VFA among LMA, MMA and HMA were not significant. Molar proportion of acetate was not affected significantly, whereas those of propionate and butyrate were linearly increased with increase in MA supplementation. As a consequence, the ratio of acetate to propionate was linearly reduced. Ruminal ammonia N and lactate content was reduced either linearly or quadratically with increase in MA supplementation.
Effects of malic acid supplementation on ruminal pH and fermentation in steers

VFA = volatile fatty acid.
aControl (without malic acid), LMA (malic acid-low), MMA (malic acid-medium) and HMA (malic acid-high) with 0.0, 7.8, 15.6 and 23.4 g malic acid per kg dry matter, respectively.
Effective ruminal degradability
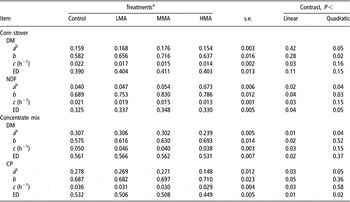
In situ ruminal digestion kinetics and ED of corn stover and concentrate mix are shown in Table 3. For corn stover, the soluble fraction of DM was quadratically changed, whereas a quadratical increase in ruminal potentially degradable fraction and a linear decrease in degradation rate were observed with increase in MA supplementation. The ED of DM was not affected significantly by MA supplementation. Regarding the digestion kinetics of NDF, the soluble fraction was linearly increased and the potential degradable fraction was linearly and quadratically changed with increasing dose of MA supplementation. The degradation rate was linearly decreased with increasing dose of MA supplementation. The ED of NDF was linearly and quadratically increased with increase in dose of MA supplementation.
In situ ruminal digestion kinetics and effective degradability of corn stover and concentrate mix

DM = dry matter; ED=effective degradability; NDF = neutral detergent fiber.
aControl (without malic acid), LMA (malic acid-low), MMA (malic acid-medium) and HMA (malic acid-high) with 0.0, 7.8, 15.6 and 23.4 g malic acid per kg dry matter, respectively.
bParameters were calculated from the fitted equation y = a + b(1−e−c(t−L)) for t > L, where y = percentage of DM disappearance from the nylon bag at time t, a = soluble fraction, b = slowly degradable fraction, c = fraction rate constant at which b is degraded, L = lag time (hours), and t = time of incubation (hours). ED was calculated using equation a + bc/(c + k), where k = 0.025 or 0.058 h−1 for corn stover or concentrate mix, respectively.
For the concentrate mix, the soluble fraction, rate of degradation and ED of DM decreased linearly, but the potentially degradable fraction increased linearly with increasing doses of MA supplementation. Similarly, the soluble fraction, rate of degradation and ED of crude protein (CP) decreased linearly, but the potentially degradable fraction increased linearly with increasing dose of MA supplementation.
Urinary purine derivatives
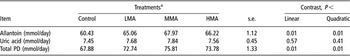
Urinary PDs are shown in Table 4. Daily urinary excretion of uric acid was not affected by the treatments, but urinary excretion of allantoin and PD (mmol/day) was affected quadratically by MA supplementation, being highest for MMA (75.81) and HMA (73.78), and lowest for control (67.88) and intermediate for LMA (72.74).
Effects of malic acid on urinary excretion of purine derivatives in steers

PD = purine derivative.
aControl (without malic acid), LMA (malic acid-low), MMA (malic acid-medium) and HMA (malic acid-high) with 0.0, 7.8, 15.6 and 23.4 g malic acid per kg dry matter, respectively.
Digestibility in the total tract
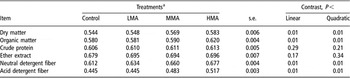
Nutrient digestibilities in the total tract are shown in Table 5. Digestibilities of DM, OM and fiber in the total tract responded linearly to MA supplementation. The digestibilities of DM, OM, NDF and ADF were linearly increased with increasing dose of MA supplementation, but the digestibilities of CP and ether extract (EE) were not affected by MA supplementation.
Effects of malic acid supplementation on nutrient digestibility in the total tract of steers

aControl (without malic acid), LMA (malic acid-low), MMA (malic acid-medium) and HMA (malic acid-high) with 0.0, 7.8, 15.6 and 23.4 g malic acid per kg dry matter, respectively.
Discussion
Ruminal fermentation
Supplementation of MA in the diet of steers altered rumen fermentation pattern from acetate to propionate production as shown in the linear reduction in the ratio of acetate to propionate with increasing MA doses (Table 2). By increasing the doses of MA supplementation, the reduction in the ratio of acetate to propionate resulted from increase in molar proportion of propionate. Furthermore, the increase in total VFA concentration was due to the significantly increased propionate and butyrate concentration. It is suggested that MA supplementation in corn stover-based diets fed to steers changed microbial composition. This is consistent with the study of Kung et al. (Reference Kung, Huber, Krummrey, Allison and Cook1982) who reported that MA supplementation increased total VFA concentration. Similarly, Martin and Streeter (Reference Martin and Streeter1995) found MA supplementation increased the concentrations of propionate and total VFA by stimulating the in vitro mixed ruminal microorganism fermentation. Martin et al. (Reference Martin, Sullivan and Evans2000) observed that sugars plus MA treatment increased concentrations of acetate, propionate and total VFA. Gómez et al. (Reference Gómez, Tejido and Carro2005) reported the addition of MA to medium- and high-concentrate diets increased the production of propionate and butyrate. However, Martin et al. (Reference Martin, Streeter, Nisbet, Hill and Williams1999) observed that ruminal pH and acetate increased, and total VFA decreased with increasing doses of MA supplementation. Carro et al. (Reference Carro, Ranilla, Giráldez and Mantecón2006) reported that MA addition increased the molar proportion of ruminal butyrate significantly. Sniffen et al. (Reference Sniffen, Ballard, Carter, Cotanch, Danna, Grant, Mandebvu, Suekawa and Martin2006) observed that MA supplementation did not affect the production of total VFA, propionate, butyric acid, the ratio of acetate to propionate, or pH. These inconsistent responses could be related to the different experimental conditions found in vivo and in vitro. In vivo, the ruminal DM content ranged from 10% to 25%, whereas in vitro, the DM content of digesta represented about 2% to 4% of the total volume. When concentrations of MA are expressed as g/g DM, marked differences between experiments were observed. In the in vitro experiments with batch cultures (Callaway and Martin, Reference Callaway and Martin1996; Carro and Ranilla, Reference Carro and Ranilla2003; Tejido et al., Reference Tejido, Ranilla, García-Martinez and Carro2005), 4, 8 and 12 mM MA represented, respectively, 6.8%, 12.7% and 17.1% of incubated substrate (DM basis). However, MA concentrations in vivo were much lower and ranged from 0.28% to 1.6% of the total diet DM (Martin et al., Reference Martin, Streeter, Nisbet, Hill and Williams1999). In this study, MA concentrations (DM basis, ranged from 0.78% to 2.34%) were higher than previous in vivo studies. In addition, the quadratic response to the dose of MA supplementation indicated that further increase of MA dose from 15.6 to 23.4 g/kg DM was not beneficial to increase the total VFA concentration and the proportion of propionate (Table 2). It is suggested that MA could selectively stimulate or inhibit the activity of ruminal microbes at certain concentrations.
Ruminal lactate content was reduced either linearly or quadratically with increasing MA supplementation. This is consistent with Castillo et al. (Reference Castillo, Benedito, Pereira, Vázquez, López Alonso, Méndez and Hernández2007) who observed that MA supplementation did decrease the l-lactate concentrations in blood. Similarly, Sniffen et al. (Reference Sniffen, Ballard, Carter, Cotanch, Danna, Grant, Mandebvu, Suekawa and Martin2006) reported that MA supplementation at 50 g/cow per day had the lowest lactic acid production. However, Streeter et al. (Reference Streeter, Nisbet, Martin and Williams1994) observed that MA supplementation (80 g/day) had very little effect on ruminal lactate concentrations. Montaño et al. (Reference Montaño, Chai, Zinn-Ware and Zinn1999) observed that MA supplementation had no effects on ruminal dl-lactate concentrations after glucose infusion in Holstein steers. It is believed that ionophores are effective in reducing the incidence of acidosis by decreasing lactate production and increasing pH within the rumen (Dennis et al., Reference Dennis, Nagaraja and Bartley1981; Russell and Strobel, Reference Russell and Strobel1989). A different mechanism seems to be involved with MA, rather than decreasing lactate production like the ionophores, MA stimulates lactate utilization by Selenomonas ruminantium HD4 (Linehan et al., Reference Linehan, Scheifinger and Wolin1978; Nisbet and Martin, Reference Nisbet and Martin1993) and a recent ruminal selenomonad isolate, strain H18 (Strobel and Russell, Reference Strobel and Russell1991). Nisbet and Martin (Reference Nisbet and Martin1991) reported that lactic acid uptake and utilization by S. ruminantium was stimulated in the presence of MA. The stimulatory effects of MA on lactic acid fermentation have been clearly demonstrated in vitro (Nisbet and Martin, Reference Nisbet and Martin1994; Martin and Streeter, Reference Martin and Streeter1995; Callaway and Martin, Reference Callaway and Martin1996). Nevertheless, there is mounting evidence that the effect of MA on lactic acid utilization may largely depend on the general nature of the substrate and the stage of fermentation. Nisbet and Martin (Reference Nisbet and Martin1994), for example, observed that the stimulatory effects of MA on lactate utilization were inhibited when cultures were grown on soluble carbohydrate.
In situ ruminal degradability and apparent digestibility in the total tract
The linear increase of in situ ruminal ED of corn stover DM and NDF was consistent with linearly increased ruminal total VFA concentration (Table 2) by increasing the dose of MA supplementation. Furthermore, the linear responses of ED of corn stover DM and NDF also supported the results of linearly increased nutrient digestibility in the total tract with MA supplementation. It is suggested that the improvement of the total digestibilities of DM, NDF and ADF due to MA supplementation was partially attributed to improved ruminal degradation. The increased in situ ruminal fiber digestibility in the present study is in agreement with other in vitro studies that ruminal fiber digestion is enhanced by additional MA (Carro et al., Reference Carro, López, Valdés and Overjero1999; Carro and Ranilla, Reference Carro and Ranilla2003). Similarly, Martin et al. (Reference Martin, Streeter, Nisbet, Hill and Williams1999) found that feed efficiency and ADG linearly increased with 80 g/day dl-MA. In semi-continuous culture systems (Gómez et al., Reference Gómez, Tejido and Carro2004), DM and NDF digestibility was higher when diets (60 : 40 and 10 : 90 forage-to-concentrate ratio) were supplemented with 6.65 mM MA. Gómez et al. (Reference Gómez, Tejido and Carro2005) found that MA treatment increased DM, NDF and ADF disappearance after 48-h incubation. Whereas adding MA to the medium-concentrate diets produced the growth of solid-associated microorganisms, no effects were observed for high-concentrate diets. Sniffen et al. (Reference Sniffen, Ballard, Carter, Cotanch, Danna, Grant, Mandebvu, Suekawa and Martin2006) reported that the digestibility of ADF and NDF was higher (P < 0.05) when MA was supplemented at 100 g/cow per day compared to 0 g/cow per day. However, other studies did not find evidence of feeding MA on improving ruminal digestibility. Montaño et al. (Reference Montaño, Chai, Zinn-Ware and Zinn1999) reported that MA supplementation did not affect ruminal digestion of OM or ADF in steers fed an 81% steam-flaked barley-based diet. Carro et al. (Reference Carro, Ranilla, Giráldez and Mantecón2006) reported that MA supplementation (4 or 8 g/kg of concentrate in Merino lambs) had no effects of MA on concentrate or straw intake, ADG, and apparent digestibility of OM, CP, NDF or ADF. One can suggest that inconsistent responses could be due to the different ratio of forage to concentrate, the digestion of nutrient increased with the increase in the ratio of forage to concentrate and the dose of MA.
Moreover, it is also suggested that MA improved nutrient digestibility in the intestine since the percent units increased for the total digestibilities of DM or NDF were greater than those reported for in situ ruminal ED. Improved animal growth rate and feed efficiency likely resulted from increased nutrient digestibility in the digestive tract with MA supplementation. The quadratic response to MA supplementation with no further improvement of in situ ruminal degradation and total digestibility is consistent with results that indicate rumen fermentation with high dose of MA supplementation (23.4 g/kg DM) was not beneficial. This further suggested that MA modulates the digestive microorganisms or enzymes in a quadratic pattern.
N metabolism and PD excretion
The increased urinary excretion of PD (Table 4) suggested that the microbial protein production in the rumen would be increased with MA supplementation. The linear reduction in ruminal ammonia N concentration could be related to an energy : N balance effect increasing microbial protein formation. Cellulolytic bacteria derive their N exclusively from ammonia N (Russell et al., Reference Russell, O’Connor, Fox, Van Soest and Sniffen1992). One can suggest that MA supplementation may improve ruminal fibrolytic bacterial activity as in situ ruminal ED of NDF was linearly improved (Table 3). Nevertheless, ammonia N concentration (Table 2) was higher than 5 mg/dl, which is necessary to support optimal microbial growth (Satter and Slyter, Reference Satter and Slyter1974). This result is in agreement with the study of Sniffen et al. (Reference Sniffen, Ballard, Carter, Cotanch, Danna, Grant, Mandebvu, Suekawa and Martin2006) who reported that microbial nitrogen production and efficiency of OM and total carbohydrate use for microbial nitrogen production increased with either 50 or 100 g of supplemental MA. However, Carro et al. (Reference Carro, Ranilla, Giráldez and Mantecón2006) found that MA supplementation (4 or 8 g/kg of concentrate in Merino lambs) did not influence the daily urinary excretion of total PDs, and therefore there were no treatment effects on estimated microbial nitrogen flow at the duodenum. These inconsistent responses could be due to the different basal diet and the dose of MA. Ingredient composition of the basal diet was approximately 351 g of corn silage, 170 g alfalfa grass silage and 479 g concentrate per kg diet on a DM basis in the study of Sniffen et al. (Reference Sniffen, Ballard, Carter, Cotanch, Danna, Grant, Mandebvu, Suekawa and Martin2006); however, the basal diet in the study of Carro et al. (Reference Carro, Ranilla, Giráldez and Mantecón2006) was 500 g of barley straw and 500 g concentrate per kg diet on a DM basis. The dose of MA applied in the study of Sniffen et al. (Reference Sniffen, Ballard, Carter, Cotanch, Danna, Grant, Mandebvu, Suekawa and Martin2006) was higher than those used in the study of Carro et al. (Reference Carro, Ranilla, Giráldez and Mantecón2006). In the present study, the basal diet was 600 g of corn stove and 400 g concentrate per kg diet on a DM basis. Furthermore, the dose of MA applied in the current study was considerably higher than those used in the previous studies of Sniffen et al. (Reference Sniffen, Ballard, Carter, Cotanch, Danna, Grant, Mandebvu, Suekawa and Martin2006) and Carro et al. (Reference Carro, Ranilla, Giráldez and Mantecón2006).
Conclusion
Increasing supplementation of MA in the diet of steer linearly increased rumen VFA concentration and altered rumen fermentation pattern into more propionate production. In situ ruminal NDF degradation of corn stover was improved but the CP degradability of concentrate mix was decreased with increasing dose of MA. Urinary excretion of purine derivatives and nutrient digestibility in the total tract were also improved with MA supplementation. The results suggest that MA modulates the digestive microorganisms or enzymes in a quadratic response. The optimum MA dose was about 15.6 g/kg DM and further increase to 23.4 g/kg DM was not beneficial to improve the feed utilization in the present experimental conditions. The mode of action of MA in the digestive tract of cattle is simply an energy supply response. Further study is warranted to focus on the mechanism of MA in the digestive tract.
Acknowledgements
This work was supported by a grant from 11th Five-Year key projects of National Scientific Research Foundation of China (2007BAD5B04). The authors thank the staff of Shanxi Agriculture University Beef Unit for care of the animals.