Introduction
The Guadalupian extinction is an enigmatic crisis because of its disparate taxonomic and, potentially, its unusually large ecological effects on different marine groups. Occurring in the late part of the Capitanian stage (259 Ma [Shen et al. Reference Shen, Henderson, Bowring, Cao, Wang, Wang, Zhang, Zhang and Mu2010]), approximately 8 Myr before the end-Permian mass extinction, the crisis was severe for fusulinoidean foraminifera (Stanley and Yang Reference Stanley and Yang1994; Groves and Wang Reference Groves and Wang2013) and perhaps in reef ecosystems (Weidlich et al. Reference Weidlich, Kiessling and Flügel2003) but only caused slightly elevated taxonomic losses among most benthic marine invertebrates (Clapham et al. Reference Clapham, Shen and Bottjer2009) (Fig. 1). Despite the limited taxonomic severity, the Guadalupian extinction may have had more pronounced ecological consequences (McGhee et al. Reference McGhee, Clapham, Sheehan, Bottjer and Droser2013). Although brachiopod extinction rates were not elevated above background in equatorial regions of Tethys (Shen and Shi Reference Shen and Shi2002), Shen and Shi (Reference Shen and Shi1996) noted that dominant brachiopod genera characterizing the Guadalupian fauna in South China disappeared and were replaced by typical Lopingian dominants. On the basis of abundance counts of silicified samples from South China, Greece, and the western United States, Clapham and Bottjer (Reference Clapham and Bottjer2007a,Reference Clapham and Bottjerb) also argued for a major increase in the ecological importance of mollusks, from Guadalupian paleocommunities overwhelmingly dominated by brachiopods to Lopingian paleocommunities where mollusks constituted nearly two-thirds of all individuals.
Guadalupian–Lopingian (middle-late Permian) timescale and extinction rates. Extinction rates for marine invertebrates (solid circles) are calculated from Paleobiology Database occurrences, using the “three-timer” method (Alroy Reference Alroy2010) with genus-level data binned at stage level (Payne and Clapham Reference Payne and Clapham2012). Fusulinoidean extinction rates (open circles) are from Groves and Wang (Reference Groves and Wang2013), using the boundary-crosser method (Foote Reference Foote2000) on species-level ranges from a composite section, calculated at 500-Kyr intervals.

The precise timing of taxonomic losses and proposed ecological shifts has been constrained only to stage-level resolution, but it is plausible to infer that they were caused by the same environmental stresses that led to the extinction. The Guadalupian crisis coincided with Emeishan flood basalt eruptions (Bond et al. Reference Bond, Hilton, Wignall, Ali, Stevens, Sun and Lai2010), although climate cooling or sea-level fall have also been proposed as mechanisms (Isozaki et al. Reference Isozaki, Kawahata and Minoshima2007; Wignall et al. Reference Wignall, Vedrine, Bond, Wang, Lai, Ali and Jiang2009). Selective taxonomic survival favored mollusks over brachiopods (Clapham and Payne Reference Clapham and Payne2011; Kiessling and Simpson Reference Kiessling and Simpson2011; Bush and Pruss Reference Bush and Pruss2013), consistent with the direction of the brachiopod-mollusk ecological shift (Clapham and Bottjer Reference Clapham and Bottjer2007a,Reference Clapham and Bottjerb).
Although the Guadalupian extinction had severe ecological consequences in certain ecosystems (McGhee et al. Reference McGhee, Clapham, Sheehan, Bottjer and Droser2013), such as a major decline in reef-building, the magnitude of disruption in level-bottom communities is not well understood. The shift in dominant brachiopod genera from the Guadalupian to Lopingian in South China (Shen and Shi Reference Shen and Shi1996, Reference Shen and Shi2009) is based on qualitative assessment of relative abundance, raising doubts about its significance. Were relative-abundance changes across the Guadalupian–Lopingian (G-L) transition unusually large in comparison with other time intervals? Furthermore, is the South China record typical of broader ecological turnover or is it a local signal? The main line of evidence for ecological decoupling in level-bottom communities, the brachiopod-mollusk transition proposed by Clapham and Bottjer (Reference Clapham and Bottjer2007a,Reference Clapham and Bottjerb), was supported by quantitative abundance counts from a limited number of silicified samples. Even though those samples came from multiple geographic regions (South China, Greece, the United States, and one from Thailand), the ecological shift should also be recognizable in additional samples, including those with non-silicified preservation, to demonstrate its global significance.
Because accurate reconstruction of the severity of ecological and taxonomic changes is critical for understanding the evolution of marine ecosystems, I revisit previous claims of ecological shifts in G-L level-bottom communities by combining additional census counts with global occurrence data. I use those quantitative data sets to test (1) whether shifts in the occurrence frequencies of dominant brachiopod genera were unusually large between the Capitanian and Wuchiapingian stages relative to background turnover and (2) whether mollusks (bivalves and gastropods) increased in relative abundance across that transition, coincident with the Guadalupian extinction. Finally, I use those new constraints on the severity of level-bottom ecological changes to discuss the magnitude of environmental disruption during the Guadalupian extinction.
Methods
I reassessed the two previously documented ecological transitions (the turnover in dominant brachiopod genera in Tethys and especially South China, and the shift to molluscan dominance) using occurrence data and census abundance counts from the Paleobiology Database. Changes in the brachiopod fauna were quantified by using occurrence frequency, where an occurrence is the record of a species in a single collection’s taxonomic list and occurrence frequency is the proportion of all brachiopod occurrences represented by the genus of interest. I downloaded Guadalupian and Lopingian (Roadian–Changhsingian) brachiopod occurrences on 5 September 2014, restricting the data set to localities in Tethys and the peri-Gondwana region to avoid biases from loss of the sedimentary record in other regions (e.g., western North America or eastern Australia). The download used Paleobiology Database data services (www.paleobiodb.org/data1.1) and all R code necessary for downloads and analyses are stored at https://github.com/mclapham/guadalupian-abundance-paper. Not all regions in Tethys have continuous sampling throughout the interval, so I further downloaded brachiopod occurrences from Iran, South China, and the Salt Range of Pakistan, which have good records spanning most or all of the Guadalupian and Lopingian, and analyzed them separately. In all downloads, genera with uncertain identification (those qualified by “cf.”, “aff.”, question marks, or quotation marks) were excluded and occurrences that were not assigned to a single stage were removed. All terrestrial collections were removed. After application of the filtering criteria, the data sets contain 16,035 brachiopod occurrences in Tethys, 1175 in Iran, 4513 in South China, and 5245 in Pakistan.
I investigated temporal trends in brachiopod occurrence frequency in the Tethys-wide and three regional data sets (Iran, South China, and Salt Range) using Bray-Curtis dissimilarity (in vegan 2.0.8 [Oksanen et al. Reference Oksanen, Blanchet, Kindt, Legendre, Minchin, O’Hara, Simpson, Solymos, Stevens and Wagner2013]) in R version 3.0.1 (R Development Core Team 2013). I used analysis of similarity (ANOSIM) to test the hypothesis that Guadalupian (Roadian, Wordian, and Capitanian) and Lopingian (Wuchiapingian and Changhsingian) time intervals had significantly different brachiopod faunas. ANOSIM is a nonparametric technique that compares between- and within-group rank-order similarities to test for changes in faunal composition (Clarke Reference Clarke1993). I also tested for correlation between the occurrence frequency of a genus in one stage and its occurrence frequency in the subsequent stage to investigate faunal stability. I used Kendall’s rank-order correlation, a nonparametric method, because most genera are rare (leading to highly skewed distributions of occurrence frequency) and because sampling noise leads to uncertainty in the reliability of closely ranked genera. Small faunal change will result in common genera remaining common in the subsequent time interval (strong positive correlation) whereas faunal turnover will cause poor or an inverse correlation.
Because variations in the geographic distribution of sampling may affect apparent faunal similarity between stages, particularly given the broad geographic scope of the Tethys data set, I investigated the relationship between sampling distribution and calculated faunal similarity. Faunal dissimilarity between two stages may be artificially elevated if samples from those stages come from different geographic regions. I first calculated a dissimilarity matrix (Bray-Curtis dissimilarity based on proportional occurrence frequency) comparing the brachiopod faunal composition among all stage pairs. To quantify the geographic distribution of sampling, I divided the Tethys sampling region into geographic bins and recorded the presence or absence of occurrences in each bin. This was done ten times, varying bin size from 0.5° to 5° at 0.5-degree increments, because faunal similarity decreases monotonically with distance. At each bin size, I calculated a dissimilarity matrix (Jaccard dissimilarity based on presence/absence of occurrences in geographic bins) comparing the geographic distribution of sampling among all stage pairs. Stage pairs with a similar sampling distribution will have occurrences in many of the same geographic bins. Finally, I used Mantel tests to evaluate the correlation between the faunal composition matrix and the ten sampling matrices (one at each geographic bin size).
I also downloaded census counts from 369 non-silicified Early Permian–Early Triassic fossil collections, each containing at least 30 specimens, from the Paleobiology Database on 1 September 2013. Counts pooled from multiple assemblages or beds were excluded by restricting the stratigraphic resolution to “bed” or “group of beds.” I removed collections with single-taxon counts (e.g., collections only describing brachiopods) by deleting those where the collection coverage field included “some macrofossils.” Complete download metadata are outlined in supplementary materials and the final data file is stored at https://github.com/mclapham/guadalupian-abundance-paper.
I also used occurrences as a proxy for rhynchonelliform brachiopod, bivalve, and gastropod abundance trends from the beginning of the Permian to the Middle Triassic. I downloaded Asselian–Ladinian occurrences of Rhynchonelliformea, Bivalvia, and Gastropoda from the Paleobiology Database data services on 5 September 2014. Data processing was the same as that applied to the Tethys brachiopod data set (removing collections not assigned to a stage, excluding terrestrial collections, and deleting occurrences not confidently identified at the genus level). After filtering, there are 59,523 occurrences.
Results
Brachiopod Fauna Composition
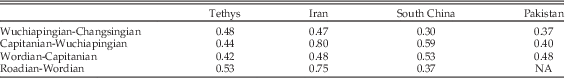
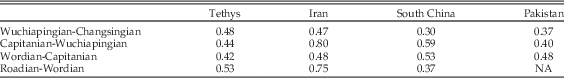
Ecological shifts triggered by the Guadalupian extinction should result in greater dissimilarity between the Capitanian and Wuchiapingian stages than between other adjacent stage pairs. The results do not clearly support that prediction; Bray-Curtis dissimilarity is not unusually elevated across the Capitanian–Wuchiapingian transition, and Capitanian and Wuchiapingian brachiopod assemblages are in fact more similar in the Tethys-wide analysis than Roadian-Wordian and Wuchiapingian-Changhsingian comparisons (Table 1). Furthermore, there is a weak but significant positive correlation between Capitanian and Wuchiapingian genus occurrence frequencies (τ=0.19), stronger than the nonsignificant correlation between Roadian and Wordian genus occurrence frequencies (τ=0.05) and similar to the Wordian-Capitanian correlation (τ=0.24), implying that the G/L boundary was not unusual compared to typical shifts in occurrence frequencies (Fig. 2). Although comparison of adjacent stages fails to reveal unusual changes at the G/L boundary, effects of the extinction may instead manifest as compositional differences between a coherent Guadalupian brachiopod fauna and a distinct Lopingian fauna. However, analysis of similarity (ANOSIM) indicates that, given stage-level variability, Guadalupian and Lopingian faunas do not form two discrete groups with distinct taxonomic compositions (R=0.67, p=0.10).
Bivariate plots showing brachiopod genus occurrence frequency (measured as the proportion of brachiopod occurrences) for successive Guadalupian-Lopingian stage pairs in the Tethyan and peri-Gondwanan region. The correlation coefficients (Kendall’s tau) above each panel are coded with significant (p<0.05) values in black and non-significant (p>0.05) values in gray.
Bray-Curtis dissimilarity values based on brachiopod occurrence frequencies for adjacent stage pairs in the entire Tethys data set and in collections from Iran, South China, and the Salt Range of Pakistan.
Although both Guadalupian and Lopingian marine deposits are found in many regions of Tethys, the spatial distribution of sampling is heterogeneous over time (Fig. 3). Except at small geographic scales, faunal dissimilarity between stages (measured with the Bray-Curtis dissimilarity index using counts of genus occurrences) is significantly correlated with sampling dissimilarity (measured with the Jaccard dissimilarity index based on presence/absence of brachiopod occurrences in geographic bins). Sampling dissimilarity measures whether the same geographic bins contain brachiopod occurrences in two different time intervals, with larger Jaccard dissimilarity values indicating sampling from different geographic regions. The degree of correlation depends on the scale of geographic binning (Fig. 4), but good correlation at scales meaningful for biogeographic provinciality (2° bins and larger, or approximately 200 km distance) implies that apparent shifts in brachiopod occurrence frequency may have been influenced, at least in part, by sampling-driven changes in the relative contribution of different regions.
Maps showing the modern geographic distribution of brachiopod occurrences used in this study. Point size is scaled to the number of occurrences at each unique latitude/longitude point.
Mantel test results indicating correlation (Spearman rho) between brachiopod faunal similarity matrix and spatial distribution of sampling matrix. Strong positive correlation at larger bin sizes indicates that time interval pairs with a more similar spatial distribution of samples tend to have more similar brachiopod faunal composition.
The influence of geographic heterogeneity in sampling can be reduced by investigating brachiopod faunal change within individual regions that have good Guadalupian and Lopingian fossil records, such as Iran, South China, and the Salt Range of Pakistan. However, Bray-Curtis dissimilarities between Capitanian and Wuchiapingian stages in those regions are not consistently greater than the dissimilarity across other stage pairs. Capitanian and Wuchiapingian brachiopod faunas in Iran were highly dissimilar, but dissimilarity was not elevated during the same interval in Pakistan (Table 1). The Roadian–Wordian transition in Iran was also marked by substantial shifts in brachiopod faunal composition, comparable with Capitanian-Wuchiapingian dissimilarity. Although end-Guadalupian abundance changes were also more pronounced in South China, their significance is not clear because the dissimilarity value was also high between the Wordian and Capitanian stages.
Comparisons of proportional genus abundance between successive stages suggest more pronounced faunal change between the Capitanian and Wuchiapingian, at least in Iran and South China (Fig. 5). In Iran, there was significant anti-correlation (τ=−0.27, p=0.007) between Capitanian and Wuchiapingian brachiopod occurrences (common Capitanian taxa were likely to be rare in the Wuchiapingian, and vice versa), whereas the correlation was significantly positive between the Wordian and Capitanian (τ=0.34, p<0.001) and weak or absent between the Roadian and Wordian (τ=0.22, p=0.051) and Wuchiapingian and Changhsingian (τ=0.15, p=0.17). Brachiopod occurrences were often significantly correlated in South China (Roadian-Wordian, τ=0.41, p=0.003; Wordian-Capitanian, τ=0.16, p=0.04; Wuchiapingian-Changhsingian, τ=0.42, p<0.001); the Capitanian-Wuchiapingian (τ=0.01, p=0.75) is the only exception. Trends differed in the Salt Range of Pakistan, however, with the Capitanian-Wuchiapingian transition actually exhibiting the strongest correlation (τ=0.44, p<0.001). Brachiopod occurrences were also significantly correlated from the Wuchiapingian to Changhsingian (τ=0.4, p<0.001) but not from the Wordian to Capitanian (τ=0.13, p=0.19). As in the Tethys-wide analysis, ANOSIM also shows that Guadalupian and Lopingian brachiopod faunas are not divided into two compositionally distinct clusters, either in Iran (R=0.83, p=0.11), South China (R=0.92, p=0.10), or Pakistan (R=0.33, p=0.50).
Bivariate plots showing brachiopod genus occurrence frequency (measured as the proportion of brachiopod occurrences) for successive Guadalupian-Lopingian stage pairs in Iran, South China, and the Salt Range of Pakistan. The correlation coefficients (Kendall’s tau) above each panel are coded with significant (p<0.05) values in black and non significant (p>0.05) values in gray.
Brachiopod-Bivalve Transition
As discussed by Clapham and Bottjer (Reference Clapham and Bottjer2007b), rhynchonelliform brachiopods were overwhelmingly dominant in silicified Guadalupian assemblages (99% of specimens in 11 samples from Nevada and Texas), but were significantly reduced in abundance in the Lopingian (only 34.6% of specimens in 12 samples from China and Greece). It is unlikely that the shift represents biogeographic variations in abundance, not only because such dramatic variations are highly implausible, but also because a silicified Guadalupian sample from Thailand exhibits similarly strong dominance by rhynchonelliform brachiopods (Clapham and Bottjer Reference Clapham and Bottjer2007b). This dramatic relative-abundance shift is not observed in non-silicified fossil collections, however, where rhynchonelliform brachiopods remained highly abundant in the Lopingian (median relative abundance of 97% in 53 samples; Fig. 6). There is considerable variability in the relative abundance of brachiopods within single fossil assemblages, in part due to lithological and latitudinal gradients and to a pronounced onshore-offshore biotic gradient (Clapham and Bottjer Reference Clapham and Bottjer2007a), but the median abundance is fairly consistent from the Cisuralian (93% of specimens based on 160 samples), Guadalupian (82% in 57 samples), and Lopingian (97% in 53 samples). In non-silicified collections, the shift in ecological dominance instead coincided with the end-Permian mass extinction when rhynchonelliform brachiopods became extremely rare (median relative abundance of 0% in 99 Early Triassic fossil assemblages) before recovering to moderate abundance in the Middle Triassic.
Box-and-whisker plots showing the proportional abundance of rhynchonelliform brachiopods in 391 Cisuralian (early Permian) to Early Triassic census counts. Solid lines indicate the median proportional abundance and boxes span the interquartile range.
Silicified and non-silicified bulk samples both potentially suffer from the same problem, that they may not be representative of globally averaged relative abundances because of limited sample size and the potential for resulting geographic, environmental, or taphonomic biases. Because abundant groups also tend to have many occurrences (Buzas et al. Reference Buzas, Koch, Culver and Sohl1982), comprehensive and global taxonomic occurrences in the PaleoDB provide a proxy for abundance that greatly reduces the likelihood of small-sample-size geographic or environmental biases. Rhynchonelliform brachiopods typically constitute 75-80% of PaleoDB brachiopod, bivalve, and gastropod occurrences during the Permian (with a range from 75.4% in the Kungurian to 84.6% in the Asselian; Fig. 7). Notably, there was no change in rhynchonelliform brachiopod occurrence frequency from the Capitanian (80.6%) to Wuchiapingian (80.8%). Bivalve and gastropod occurrence frequency also varied over a narrow range and, like rhynchonelliform brachiopods, did not change from the Capitanian to Wuchiapingian (Fig. 7). Global occurrence frequency paralleled the non-silicified abundance data and exhibited a marked shift from common rhynchonelliform brachiopods to common bivalves between the Changhsingian to Induan. All three data sets (global occurrences, non-silicified abundances, and silicified abundances) are in agreement except during the Lopingian, when silicified collections record a considerable increase in the relative abundance of mollusks, especially gastropods (Clapham and Bottjer Reference Clapham and Bottjer2007b), that is not observed in global occurrences or non-silicified collections.
Occurrence frequency (proportion of all brachiopod, bivalve, and gastropod occurrences represented by each group) for rhynchonelliform brachiopods, bivalves, and gastropods in the Permian and early Middle Triassic. Error bars are binomial confidence intervals based on the Wilson score interval. Dashed line indicates the Guadalupian extinction (near or at the end of the Capitanian stage) and the solid line indicates the end-Permian mass extinction.
Discussion
Brachiopod Faunal Composition and the Guadalupian Extinction
In many regions, Lopingian brachiopod assemblages can qualitatively be distinguished from Guadalupian assemblages, but does the evidence support significant changes in brachiopod occurrence frequencies, potentially caused by the Guadalupian extinction, beyond the expectations of background faunal turnover? The evidence from Tethys-wide data is equivocal. Bray-Curtis dissimilarity does not peak at the Capitanian-Wuchiapingian transition relative to other stages and Guadalupian and Lopingian faunas do not form significant discrete clusters according to the ANOSIM results. Although the ANOSIM results were not statistically significant using the traditional definition (p<0.05), the rank-order test has very low power to recognize significant differences with a sample size of only five time intervals. Correlations of genus occurrence frequencies are also ambiguous; the change from Capitanian to Wuchiapingian stages was slightly greater than the Wordian-Capitanian or Wuchiapingian-Changhsingian, but less than the Roadian-Wordian. Together these results could be interpreted to indicate that the G-L transition was not marked by unusually large changes in brachiopod occurrence frequency. If true, the implication is that the Guadalupian extinction did not cause major shifts in the relative abundance within brachiopod assemblages.
It is more likely, however, that Tethys-wide faunal patterns are too heavily influenced by sampling and other random noise to be meaningful, especially given that brachiopod faunal dissimilarity is significantly correlated with geographic variations in sampling (Fig. 4). Although the correlation between the two does not necessarily prove that spatially variable sampling was responsible for some of the variation in brachiopod occurrence frequency, it is plausible that sampling noise could have obscured true patterns. The strength of correlation is dependent on the scale of geographic binning and only larger scales exhibit significant correlation between faunal composition and sampling (Fig. 4), but there are two reasons to think that the stronger correlation at larger bin sizes should be a better indicator of the effects of sampling. First, small bin sizes are more likely to suffer from random sampling outages, introducing noise to the data that will artificially reduce the correlation. Second, the Jaccard coefficient is influenced by the number of shared sampled bins (where the same bin contains samples in both time intervals), without considering the geographic proximity of bins. Small-scale heterogeneity in the geographic distribution of sampling between two time intervals, which may result in high Jaccard dissimilarity, is less likely to create spurious faunal differences between those intervals because sampling may still encompass similar biogeographic regions. As long as samples come from the same general regions (e.g., South China or Iran), it matters less whether they come from a particular 30 km bin within those regions. In contrast, heterogeneity at large geographic scales (e.g., samples from one time interval come primarily from South China whereas samples from the other time interval come primarily from Iran) should have a larger effect on the faunal composition because the two faunal lists record different biogeographic regions. In that case, the correlation between high Jaccard dissimilarity and high Bray-Curtis dissimilarity may suggest that the faunal dissimilarity between those intervals is artificially elevated due to sampling biases. Geographic heterogeneity in sampling may also result in variable contributions from different facies, but that is less likely to be important with large data sets and should not vary as strongly with bin size (two collections may come from different facies regardless of whether they are separated by 50 km or 5000 km).
Because sampling variability introduces enough uncertainty to prevent reliable interpretation of the Tethys-wide results, trends from single regions (Iran, South China, and Pakistan) may provide clearer signals of brachiopod faunal change. In Iran and South China, the Capitanian-Wuchiapingian transition exhibited larger shifts in brachiopod occurrence frequencies than typical background levels, consistent with greater-than-normal faunal change. The same is not true in Pakistan, however, where the correlation between genus occurrence frequencies was actually greatest across the Capitanian/Wuchiapingian boundary, indicating that faunal shifts did not exceed background levels. Bray-Curtis dissimilarity values are also mixed; dissimilarity is elevated between the Capitanian and Wuchiapingian in Iran (but also between the Roadian and Wordian) and South China (although values are similar to the Wordian–Capitanian), but not in Pakistan. The Capitanian/Wuchiapingian boundary does not stand out as an unusual event based on Bray-Curtis dissimilarity. Finally, ANOSIM results indicate that Guadalupian and Lopingian faunas do not form discrete groups, although hypothesis testing is hindered by low statistical power and the R value is very high for the Iran (0.83, where a value of 1 indicates that all between-group distances are greater than within-group distances) and South China data sets (0.92). Together, those results suggest that moderate faunal change may have occurred within brachiopod faunas across the G/L boundary, especially in Iran and South China, but that the magnitude of change cannot clearly be distinguished from background levels.
Although regional faunal data are far less likely to be influenced by shifts in the geographic distribution of samples, facies changes can instead have important effects on faunal composition. In South China, the weaker correlation between the Wordian and Capitanian stages may in part reflect the importance of distinctive reef-associated brachiopods in the Capitanian Lengwu Formation (Liang Reference Liang1990). Analyses removing Lengwu collections emphasize Capitanian-Wuchiapingian dissimilarity, which stands out even more relative to the background of other stage transitions. The Capitanian–Wuchiapingian transition was also marked by a shift from nearly exclusively carbonate facies (Maokou and Lengwu Formations) to a mixture of carbonate (Wujiaping Formation) and siliciclastic facies (Longtan Formation). In Pakistan, however, the Wargal Formation spans the Capitanian/Wuchiapingian boundary (although not necessarily conformably) and is represented by carbonate platform settings in both stages (Mertmann Reference Mertmann2003). In contrast, Wordian and Capitanian brachiopod occurrences frequencies are not significantly correlated, coincident with a shift from the predominantly siliciclastic Amb Formation to the carbonate Wargal Formation (Mertmann Reference Mertmann2003). Facies changes in Iranian sections were less pronounced, but Wordian and Capitanian shallow-marine carbonate units in Julfa and the Alborz Mountains (Gnishik, Khachik, and Ruteh Formations) are overlain by deeper marl facies in the Wuchiapingian (Julfa and Nesen Formations) (e.g., Angiolini and Carabelli Reference Angiolini and Carabelli2010; Crippa and Angiolini Reference Crippa and Angiolini2012). Other stage transitions with substantial facies changes, like the Wuchiapingian-Changhsingian in South China (Longtan/Wujiaping to carbonate Changxing Formation) and Pakistan (shift to mixed carbonate-siliciclastic in the Chhidru Formation), nevertheless exhibit strong correlation of occurrence frequencies (Fig. 5), implying that facies changes did not necessarily cause faunal shifts.
Given these lines of evidence, did the Guadalupian extinction cause shifts in brachiopod abundances that were significantly greater than background faunal change? Tethys-wide occurrences are ambiguous because of geographic shifts in sample distribution, but data from Iran and South China suggest faunal turnover, although perhaps not much greater than background levels. It is likely that the observed faunal turnover, at least in Iran and South China, is a real phenomenon (not driven exclusively by facies changes) because facies changes are only inconsistently associated with shifts in occurrence frequency. The reasons for the discrepancy between Pakistan and Iran/South China are not clear; it could reflect geographic or environmental variations in the response to the Guadalupian extinction but the small sample size precludes firm conclusions. It is also possible that stage-level correlations are obscured by random sampling effects or other sampling biases so that the trends in any single region are not representative. Environmental stresses associated with the Guadalupian extinction may have been responsible for changes in brachiopod abundances, but other stages also exhibit changes of similar magnitude.
Timing of the Brachiopod-Bivalve Transition
The silicified samples examined by Clapham and Bottjer (Reference Clapham and Bottjer2007b) recorded a major increase in the abundance of mollusks between the Capitanian and Wuchiapingian, which would indicate significant ecological consequences of the Guadalupian extinction if the abundances reflect global patterns. However, the fact that non-silicified samples and global occurrence data do not display the same increase in molluscan dominance raises doubts about the silicified record. Although it is possible that neither record is accurate, the most likely options are (1) silicified assemblages more accurately record global abundances because of biases in non-silicified assemblages or (2) non-silicified assemblages are a better record because of small sample size or other biases in the silicified collections.
Option 1: The Silicified Record Is More Accurate
The loss of aragonitic fossils during early diagenesis and the consequent overrepresentation of calcite-shelled species in paleontological samples has been well documented (Cherns and Wright Reference Cherns and Wright2009). Many Permian bivalves and nearly all gastropods had aragonite shells, whereas rhynchonelliform brachiopods were exclusively low-Mg calcite, implying that the vast majority of Permian fossil assemblages should be artificially mollusk-poor because of diagenetic aragonite dissolution. Silicified assemblages, especially samples where silicification occurred early during diagenesis prior to aragonite dissolution, are therefore more likely to capture the true biotic composition. Textural evidence suggests that silicification was an early diagenetic phenomenon in the samples examined by Clapham and Bottjer (Reference Clapham and Bottjer2007b), so it is possible that increased molluscan dominance reflects a true ecological shift during the Guadalupian extinction.
The ease of extracting fossils from silicified samples by acid dissolution also enables identification and counting of extremely small specimens that would otherwise be difficult to recognize. In the Clapham and Bottjer (Reference Clapham and Bottjer2007b) samples, that smallest size-fraction was strongly dominated by gastropods, and the ability to identify and count numerous 2–5-mm-high gastropod shells (Clapham and Bottjer Reference Clapham and Bottjer2007a) greatly increased the abundance of mollusks in many of the samples. Those tiny shells may not be recognizable in non-silicified samples where mechanical disaggregation is the only method of counting, or may not even be preserved following aragonite dissolution during diagenesis (which is likely to affect small shells more severely). Because gastropods often dominate the smaller size-fractions, counting only larger shells that may be identifiable in non-silicified samples will bias estimates of numerical dominance toward brachiopods. For that reason, silicified samples may be a more accurate representation of the original community and therefore a better record of changes in abundance over time.
Option 2: The Non-Silicified Record is More Accurate
Although silicified fossil assemblages have several advantages described above, the samples described by Clapham and Bottjer (Reference Clapham and Bottjer2007b) may not necessarily provide a more accurate record of faunal changes. Silicification was a rare phenomenon in the Guadalupian and Lopingian and can exhibit fabric selectivity (preferentially silicifying certain types of shell mineralogy or ultrastructure) or occur only in certain depositional settings (e.g., Schmitt and Boyd Reference Schmitt and Boyd1981; Erwin and Kidder Reference Erwin and Kidder2000). Those biases will be averaged by extensive sampling, but the small sample sizes (11 Guadalupian samples from Nevada and 12 Lopingian samples from China and Greece) used by Clapham and Bottjer (Reference Clapham and Bottjer2007b) may therefore not be representative of global abundances. For example, poor silicification of bryozoans in Nevada (Guadalupian), where only zooid chambers are infilled by silica, contrasts with complete silicification of branching forms in China and Greece and suggests that fabric selectivity may differ among the samples.
Early silicification is more likely to preserve aragonitic taxa, but the relative timing of silicification and aragonite dissolution is difficult to pinpoint and may have had significant effects on Guadalupian and Lopingian data. Even though silicification occurred early during sediment compaction, there were no gastropods preserved among several thousand specimens in Guadalupian samples from Nevada (Clapham and Bottjer Reference Clapham and Bottjer2007b). It is possible that no gastropods lived in the original communities, but that seems unlikely, and their absence suggests that aragonite dissolution may have occurred even earlier than silicification during diagenesis, perhaps even on the seafloor.
Non-silicified abundance counts also suffer from small sample sizes and related potential habitat, geographic, or taphonomic biases, at least in practice, because of the paucity of studies that have collected whole-assemblage counts in the Permian. Occurrences, however, are global in scope and sample thousands of fossil assemblages, greatly reducing the effects of environmental and geographic variations in abundance. Bivalve fossil abundance should also have increased if there were greater numbers of calcite-shelled or bimineralic individuals in life assemblages, unless aragonite loss became more severe in the Lopingian to offset that increase. Trends in molluscan abundance through the Early and Middle Triassic are also better interpreted as true shifts in abundance (with the caveat that mollusks are routinely underrepresented) rather than variations in aragonite dissolution, implying that the G-L record provides reliable information about relative trends in abundance.
For those reasons, it seems most likely that G-L changes in the relative abundance of rhynchonelliform brachiopods and mollusks were minimal, as indicated by the global occurrence and non-silicified counts, and that abundance shifts in existing silicified count data instead reflect different fabric selectivity or variations in the timing of silicification and aragonite dissolution in a small number of samples. The results here do not rule out changes in relative abundance, but any shift toward increased molluscan dominance was likely to have been small. The end-Permian mass extinction was instead the primary trigger of the rise of mollusks to numerical dominance (Gould and Calloway Reference Gould and Calloway1980; Fraiser and Bottjer Reference Fraiser and Bottjer2007).
Implications for the Guadalupian Extinction
Extinction events are by definition marked by elevated taxonomic losses, but can also cause ecological shifts (Droser et al. Reference Droser, Bottjer, Sheehan and McGhee2000; McGhee et al. Reference McGhee, Clapham, Sheehan, Bottjer and Droser2013). Ecological changes across the G/L boundary, such as an increase in the relative abundance of bivalves and gastropods, have previously been interpreted as an example of ecological shifts triggered by the Guadalupian extinction (Clapham and Bottjer Reference Clapham and Bottjer2007a,Reference Clapham and Bottjerb). The analyses presented here imply that there was actually little change in the relative abundances of brachiopods and mollusks across the G/L boundary. A shift in dominant brachiopod genera appears robust, at least in Iran and South China, but it may have been only slightly more pronounced than background ecological shifts between other Permian stages.
The subtle ecological changes documented here, combined with minimally elevated extinction rates among marine invertebrates (Clapham et al. Reference Clapham, Shen and Bottjer2009), suggest a minor taxonomic and ecological crisis in level-bottom habitats. The fossil record documents a continuum of faunal change, from local restructuring without extinction (e.g., Fall and Olszewski Reference Fall and Olszewski2010) to the biggest mass extinctions with catastrophic taxonomic losses and ecosystem disruption. Those biotic shifts occurred in response to environmental changes, also of varying type and magnitude, providing opportunities to investigate the relationship between environment and community ecology at a variety of scales. Although slightly elevated extinction rates and minor ecological changes may not require large environmental perturbations near the G/L boundary, it is nevertheless informative to consider whether sea-level change (Wignall et al. Reference Wignall, Vedrine, Bond, Wang, Lai, Ali and Jiang2009), climate cooling (Isozaki et al. Reference Isozaki, Kawahata and Minoshima2007), or the Emeishan flood basalts (Bond et al. Reference Bond, Hilton, Wignall, Ali, Stevens, Sun and Lai2010) were plausible triggers of ecological shifts. Guadalupian-Lopingian carbon- and calcium-cycle perturbations were weak (Jost et al. Reference Jost, Mundil, He, Brown, Altiner, Sun, DePaolo and Payne2014), implying that Emeishan volcanism did not have significant environmental effects at a global scale, consistent with the limited severity of the biotic consequences. Enriched carbon isotope values have been interpreted as a signal of enhanced organic carbon burial (in absolute terms) and therefore climate cooling (Isozaki et al. Reference Isozaki, Kawahata and Minoshima2007), but only indicate an elevated fraction of carbon buried as organic carbon and can have other explanations (Kump and Arthur Reference Kump and Arthur1999; Schrag et al. Reference Schrag, Higgins, Macdonald and Johnston2013). Sea-level change is unlikely to trigger significant extinction; however, ecological changes in level-bottom communities across the G/L boundary were subtle and it is possible that fluctuating sea level could have led to shifts in dominant genera (e.g., Brett Reference Brett1998). Shen and Shi (Reference Shen and Shi2009) described a brachiopod fauna with a mixed G-L faunal character from the latest Capitanian sea-level lowstand at Penglaitan in South China, although genera typical of the Lopingian were already dominant. That observation places preliminary constraints on the timing of the brachiopod transition, but additional samples are required to resolve its relationship to sea-level fall or other proposed environmental triggers.
Conclusions
Previous studies have argued that the Guadalupian extinction triggered unusually large ecological changes, such as a shift from brachiopod to mollusk dominance, but combined evidence from silicified and non-silicified assemblages and from global occurrences implies that the apparent brachiopod-mollusk shift more likely reflects taphonomic biases among the silicified samples rather than a global paleoecological change. Mollusks, especially bivalves, instead became numerically dominant following the end-Permian mass extinction.
Although brachiopod and mollusk relative abundances did not change substantially across the G/L boundary, the transition was marked by paleoecological changes at lower taxonomic levels within brachiopod faunas. Common Capitanian genera became rare or went extinct and were replaced by new dominant genera in the Wuchiapingian. The magnitude of faunal change between the Capitanian and Wuchiapingian may have been slightly greater than between other time intervals, but the shift was not pronounced overall and was most recognizable in Iran and South China.
Because paleoecological changes in level-bottom communities were restricted to shifts in brachiopod genus dominance while abundances of higher-level groups like brachiopods and mollusks remained largely unchanged, there is little evidence for severe ecological consequences during the Guadalupian extinction. Taxonomic losses among level-bottom invertebrates were only minimally elevated and paleoecological changes were comparably subtle. Paleoecological shifts do not help discriminate between proposed causal mechanisms, but biotic evidence and geochemical constraints suggest that there may be no need to invoke a major environmental perturbation for the Guadalupian event.
Acknowledgments
I thanks A. Bush, T. Olszewski, and J. Payne for their helpful reviews. This is Paleobiology Database contribution 208.
Supplementary material
Supplemental materials deposited at Dryad: 10.5061/dryad.rh29r