Introduction
The Hooded Grebe Podiceps gallardoi has suffered a drastic 80% decline in its population since the 1980s, with a global population now amounting to only c.700 adult individuals (Roesler et al. Reference Roesler, Imberti, Casañas, Mahler and Reboreda2012a, Reference Roesler, Lancelotti, Gabarain, Buchanan, Hernández, Fasola and Schulenberg2025). It is classified as “Critically Endangered” (BirdLife International 2023), and because of its acute and steep decline and evolutionary history, it is classified as 20th among the more than 10,000 species of birds in the EDGE of Existence Bird List (EDGE-ZSL 2023). The Hooded Grebe is an endemic breeder in southernmost continental Patagonia, Argentina (Roesler et al. Reference Roesler, Lancelotti, Gabarain, Buchanan, Hernández, Fasola and Schulenberg2025), with regular – but scattered – records in Chile, where no reproduction has yet been recorded (Roesler Reference Roesler2015).
Several threats have been identified at the Hooded Grebe’s reproductive grounds in the lakes of highland basaltic plateaus of western Santa Cruz Province, Argentina. Population viability is affected by alien invasive species, such as American mink Neogale vison (Fasola and Roesler Reference Fasola and Roesler2018; Roesler et al. Reference Roesler, Imberti, Casañas and Volpe2012b) and rainbow trout Oncorynchus mykiss (Lancelotti et al. Reference Lancelotti, Marinone and Roesler2016; Porcel et al. Reference Porcel, Fogel, Izaguirre, Roesler and Lancelotti2022), and by the neo-native Kelp Gull Larus dominicanus (Roesler et al. Reference Roesler, Fasola, Casañas, Hernández, De Miguel and Giusti2016), as well as by abiotic factors arising from global climate change (Lancelotti et al. Reference Lancelotti, Pessacg, Roesler and Pascual2020; Roesler et al. Reference Roesler, Imberti, Casañas, Mahler and Reboreda2012a). Also, projected infrastructure constructions, such as hydroelectric dams and wind farms, will affect its wintering grounds (Roesler et al. Reference Roesler, Lancelotti, Gabarain, Buchanan, Hernández, Fasola and Schulenberg2025).
The Hooded Grebe was only discovered and formally named 50 years ago (Rumboll Reference Rumboll1974). One of the reasons for this late discovery is that its main reproductive habitat is restricted to 11 isolated, remote, and almost inaccessible, highland basaltic plateaus, in western Santa Cruz Province, southern Argentina, and only a few lakes in the Magallanes Region, in extreme southern Chile (Roesler et al. Reference Roesler, Lancelotti, Gabarain, Buchanan, Hernández, Fasola and Schulenberg2025). These plateaus are island-like habitats, surrounded by deep, glacial valleys (Mazzoni and Rabassa Reference Mazzoni and Rabassa2018). For similar reasons, remoteness and the extreme conditions of the area, its migratory behaviour towards wintering grounds in estuaries of the Atlantic Ocean was only described 20 years after the discovery of the species (Johnson and Serret Reference Johnson and Serret1994). In winter, Hooded Grebes flock in the estuaries of four rivers (i.e. Coyle, Gallegos, and Santa Cruz-Chico) that flow into the Atlantic Ocean in eastern Santa Cruz Province, where groups of several hundred – up to 97% of the population – have been recorded (Roesler et al. Reference Roesler, Lancelotti, Gabarain, Buchanan, Hernández, Fasola and Schulenberg2025).
Both reproductive and wintering grounds are clearly defined and non-overlapping, which led to the idea of isolated populations (Roesler Reference Roesler2016). Furthermore, Fjeldså (Reference Fjeldså1986) suggested the probable existence of philopatry (site fidelity) in breeding populations. This behaviour seems to be supported by a relatively constant number of individuals at each plateau in different years and by regular re-observation of banded individuals (Roesler et al. Reference Roesler, Lancelotti, Gabarain, Buchanan, Hernández, Fasola and Schulenberg2025).
Genetic markers can be used to infer the connectivity among populations without the need for the logistically expensive capture, banding, and recapture (DeSaix et al. Reference DeSaix, Bulluck, Eckert, Viverette, Boves and Reese2019; Ruegg et al. Reference Ruegg, Anderson, Paxton, Apkenas, Lao and Siegel2014). In migratory species, populations are more difficult to define because individuals may share common areas at some period of their annual movements cycle (Møller et al. Reference Møller, Jokimäki, Skorka and Tryjanowski2014). However, the subdivision into reproductively isolated populations can occur despite the high mobility when individuals are philopatric and consistently return to a certain area. In some species site fidelity can be maintained both in reproductive and wintering grounds, while in others that separation is only maintained during a certain time in the annual cycle, with individuals of different populations coexisting during the rest of the year (Esler Reference Esler2000).
Migratory species are particularly susceptible to environmental changes as they depend on both wintering and reproductive areas, along with stop-over sites during migration (Runge et al. Reference Runge, Martin, Possingham, Willis and Fuller2014). Understanding the role of seasonal migration in mediating gene flow among populations is important to identify distinct evolutionary and demographic units relevant to conservation and management (Battey et al. Reference Battey, Linck, Epperly, French, Slager and Sykes2018), and to identify the impact of local stressors on population declines as disturbances at one stage of the annual cycle can have carry-over effects to other phases of the annual cycle (Kramer et al. Reference Kramer, Andersen, Buehler, Wood, Peterson and Lehman2018; Norris and Taylor Reference Norris and Taylor2006). Furthermore, restricted gene flow can accelerate the evolution of adaptive divergence (Rolshausen et al. Reference Rolshausen, Segelbacher, Hobson and Schaefer2009). This is particularly relevant in a context of climate change and high biodiversity loss (Díaz et al. Reference Díaz, Settele, Brondízio, Ngo, Agard and Arneth2019).
Here we investigated if Hooded Grebes are philopatric towards their breeding plateaus by studying their genetic population structure. This work seeks to understand populations throughout the full annual cycle, which is critical for understanding the ecology and evolutionary biology (Faaborg et al. Reference Faaborg, Holmes, Anders, Bildstein, Dugger and Gauthreaux2010; Marra et al. Reference Marra, Cohen, Loss, Rutter and Tonra2015; Sherry Reference Sherry2018), as well as detecting the potential impact of local extinctions at individual plateaus for the conservation of this Critically Endangered species. The identification of demographically independent units (Palsbøll et al. Reference Palsbøll, Berube and Allendorf2007), also called “management units” or “conservation units”, is essential to maintain the adaptive potential of threatened species and address appropriate conservation and management strategies (Allendorf and Luikart Reference Allendorf and Luikart2007; Fraser and Bernatchez Reference Fraser and Bernatchez2001). The results obtained provide key information to define and optimise present and future conservation actions of the Hooded Grebe’s Conservation Project (led by the Programa Patagonia of Aves Argentinas/BirdLife International).
Methods
Study site and species
Study site
A series of 11 highland plateaus run parallel to the Andes mountain ridge in central-western Santa Cruz Province, Argentina. Seven of those plateaus were used by the Hooded Grebe during the last 15 breeding seasons (Roesler et al. Reference Roesler, Lancelotti, Gabarain, Buchanan, Hernández, Fasola and Schulenberg2025; Figure 1A). These plateaus comprise a vast area, covering approximately 24,000 km2. The origin of the plateaus is recent from a geological point of view, since they originated during the Miocene to Pliocene geological epochs, with recent lava records of just over 100,000 years, during the Pleistocene (Brown et al. Reference Brown, Singer and Gorring2004; Lancelotti Reference Lancelotti2009; Mazzoni and Rabassa Reference Mazzoni and Rabassa2018). All plateaus are similar, although they vary in size (from 1,706 km2 to 2,983 km2). Their height ranges from 500 m to 1,500 m a.s.l., with peaks such as Mount Zeballos at 2,700 m a.s.l. (Roesler Reference Roesler2016). Most of the remaining populations of Hooded Grebes are concentrated on three of these plateaus (Roesler et al. Reference Roesler, Imberti, Casañas, Mahler and Reboreda2012a): Lake Buenos Aires Plateau (BAP) 47°09’20S 71°16’32W; Lake Strobel Plateau (ST) 48°28’40S 71°22’46W); La Siberia – or Lake San Martín – Plateau (SIB) 49°01’31S 71°43’59W) (Figure 1A).
Molecular marker distribution among plateaus: (A) mtDNA data (353 bp control region fragment); (B–D), genomic data (1,738 SNPs). (A) Circles show haplotype (H1–H11) frequency distribution among plateaus. Numbers indicate plateaus where Hooded Grebes breed (studied plateaus are coloured). 1: Buenos Aires (BAP; blue; n = 27); 2: Asador; 3: Strobel (ST; red; n = 24); 4: Ventana; 5: Moro; 6: La Siberia (SIB; green; n = 20); 7: Viedma; 8: La Gringa; 9: Vizachas; 10: La Torre. Letters indicate the estuaries where Hooded Grebes winter. A: Gallegos; B: Coyle; C: Santa Cruz; D: San Julián. (B) Principal Component Analysis; (C) Bayesian clustering; (D) Discriminant Analysis for 63 individuals (BAP, blue, n = 21; ST, red, n = 24; SIB, green; n = 18).

Study species
Although the reproductive strategy of the Hooded Grebe is somewhat similar to that of other grebes in terms of colonial behaviour, it is more extreme, forming larger, denser colonies of up to 100 pairs on just a few lakes per plateau (Beltrán et al. Reference Beltrán, Bertonatti, Johnson, Serret and Sutton1992; Fjeldså Reference Fjeldså2004; Johnson Reference Johnson1997; Roesler et al. Reference Roesler, Imberti, Casañas, Mahler and Reboreda2012a, Reference Roesler, Lancelotti, Gabarain, Buchanan, Hernández, Fasola and Schulenberg2025). This strategy facilitates the annual location of most individuals at each plateau (Roesler et al. Reference Roesler, Imberti, Casañas, Mahler and Reboreda2012a, Reference Roesler, Lancelotti, Gabarain, Buchanan, Hernández, Fasola and Schulenberg2025) during the reproductive season (October–March). Regular censuses showed relatively constant numbers at each important reproductive plateau (BAP, ST, and SIB) leading to the hypothesis that those numbers might be a consequence of a strong philopatric behaviour (Roesler Reference Roesler2016, Reference Roesler, Lancelotti, Gabarain, Buchanan, Hernández, Fasola and Schulenberg2025) with grebes returning to the same plateau after wintering in the Atlantic estuaries.
Sampling methods
Samples were obtained from a total of 71 individuals BAP (n = 27), ST (n = 24), and SIB (n = 20) (see Supplementary material Table S1). They were mostly taken during banding captures that took place in the reproductive season at night using a small net, flashlights, and an inflatable paddle boat, as described in Roesler (Reference Roesler2016) (Permit: Consejo Agrario provincial Nº31/2012-2016). A blood sample of approximately 50 μl was taken from the brachial vein and stored in lysis buffer (100 mM TRIS, 100 mM EDTA, 10 mM NaCl, 2% SDS) at room temperature until genetic analysis. Some samples were obtained from dead individuals found at the reproductive plateaus. Pectoral muscle samples of these individuals were stored in DMSO buffer (20% v/v DMSO, 250 mM EDTA, NaCl).
DNA sequencing
We purified genomic DNA from the blood samples using a DNA blood and tissue extraction kit (Qiagen, Valencia, CA, USA). A 353-bp fragment of the mtDNA control region was amplified using primers CR3F (5’ GCCYCTTATGTCGCCATGC 3’) and CR550R (5’ GGTGTAGGGGGAAAGAATGATCC 3’) (Ogawa et al. Reference Ogawa, Pulgarin, Vance, Fjeldså and van Tuinen2015). Amplification products were sequenced in an ABI 3130xl (Applied Biosystems, Foster City, CA, USA) sequencer using ABI Big DyeTM Terminator Chemistry at the Faculty of Exact and Natural Sciences, University of Buenos Aires. Sequences were edited and aligned using Clustal W (Thompson et al. Reference Thompson, Higgins and Gibson1994) with Bioedit v.7.2.5 (Hall Reference Hall1999).
We also generated restriction site-associated DNA markers using the 3RADseq procedure following Hoffberg et al. (Reference Hoffberg, Kieran, Catchen, Devault, Faircloth and Mauricio2016). The procedure was divided into two phases. First, we sequenced three individuals from different localities using 300-bp paired-end reads on the Illumina MiSeq to generate high-quality reference libraries. This followed our approach for constructing single-copy orthologs without a high-quality reference genome (Driller et al. Reference Driller, Arantes, Vilaça, Carrasco-Valenzuela, Heeger and Mbedi2021; Vilaça et al. Reference Vilaça, Maroso, Lara, de Thoisy, Chevallier and Arantes2023). Next, we prepared libraries of individual pools, calibrated via a spike-in on the Illumina MiSeq (Arantes et al. Reference Arantes, Caccavo, Sullivan, Sparmann, Mbedi and Höner2023). In short, genomic DNA of each sample was standardised to 20 ng/μl and digested using three restriction enzymes, XbaI, EcoRI, and NheI (New England Biolabs, Ipswich, MA, USA). Fragments were then ligated to P1 and P2 adapters (with unique barcode combinations) to 5’ and 3’ ends, respectively. We pooled all samples and size-selected the DNA library using BluePippin (Sage Science), retaining fragments between 290 bp and 590 bp. We then performed a single-cycle polymerase chain reaction (PCR) to add an 8N fragment at 5’ for duplicate detection and finally amplified the DNA fragments by performing eight PCR cycles with an outer P5 and an indexing P7 primer. To avoid bad sequencing outputs, we divided the library into six aliquots before performing the indexing PCR (i.e. we added six different P7 indexes). We finally pooled the six amplification products in equimolar ratios to create a single library for sequencing. The library containing 65 individuals was sequenced on one lane of an Illumina NextSeq 500 at the Berlin Center for Genomics in Biodiversity Research (BeGenDiv), producing 140 million 150-bp paired-end reads.
Bioinformatics and assembly of RAD loci
To generate the single-copy orthologs reference library based on three samples, we first improved the quality average of the 300-bp paired-end reads. Quality was assessed using FastQC version 0.11.6 and quality improvements were performed as follows. First, we cleaned fragments containing the cutting side of the third enzyme (NheI); we then trimmed Nextera Adapter Sequences with Trim Galore (Krueger Reference Krueger2021); afterwards, reads containing an average Phred quality score below 20 were removed; finally, we trimmed sequences to 220 bp using fastX_trimmer (Gordon and Hannon Reference Gordon and Hannon2010) removing shorter sequences. We demultiplexed the reads using the process_radtags module from the Stacks pipeline ver. 1.44 (Catchen et al. Reference Catchen, Hohenlohe, Bassham, Amores and Cresko2013) to obtain files containing sequences that were specific to each individual. PCR duplicates were removed using clone_filter. The single-copy orthologs reference library was built using the denovo_map.pl script from Stacks with parameters m = 3, M = 3, n = 3, and N = 5 after Paris et al. (Reference Paris, Stevens and Catchen2017). With the populations module, we retained all loci present in the three individuals (N = 20.852).
Reads obtained from the NextSeq run containing all individuals were demultiplexed using process_radtags and quality was improved as described above, with reads trimmed to 125 bp. Reads were aligned to the single-copy orthologs reference library with Bowtie2 version 2.2.8 (Langmead and Slazberg Reference Langmead and Salzberg2012) with an average alignment rate of 80%. Aligned sequences were converted with SAMtools (Li et al. Reference Li, Handsaker, Wysoker, Fennell, Ruan and Homer2009) and assembled into RAD loci using the ref_map.pl script from the Stacks pipeline (Catchen et al. Reference Catchen, Hohenlohe, Bassham, Amores and Cresko2013). Single nucleotide polymorphisms (SNPs) were then exported using the populations module, retaining loci present in at least 75% of the individuals of each plateau (r parameter) and shared among the three plateaus. We applied a minor allele frequency filter of at least 0.05 (--min_maf) and a maximum heterozygosity of 0.5 (--max_obs_het) retaining SNPs with a minimum stack depth of 10. SNPs were exported in different data sets as variant call format (.vcf).
Population genetic statistics
For mtDNA sequences, we calculated basic genetic variability parameters using the pegas package (Paradis Reference Paradis2010) in R environment (R Core Team 2017). The same package was used to analyse population structure calculating pairwise ΦST among sites.
Population genetic statistics (major allele frequency, percent polymorphic loci, nucleotide diversity (π), and Wright’s F statistics FIS) were calculated for every SNP using the populations package in Stacks (Catchen et al. Reference Catchen, Hohenlohe, Bassham, Amores and Cresko2013). We also assessed the overall level of differentiation among populations at plateaus by calculating individual (per SNP) and general (across all SNPs) differentiation (FST; Wright Reference Wright1943).
We used the R package SambaR (de Jong et al. Reference de Jong, de Jong, Hoelzel and Janke2021) to analyse population structure and population differentiation. For these analyses we exported one SNP per locus (write_single_SNP) with the populations module of Stacks. The SNP data set was converted from variant call format to the final input format with PGDSpider v.2.1.1.5 (Lischer and Excoffier Reference Lischer and Excoffier2012) and PLINK 1.9 (Chang et al. Reference Chang, Chow, Tellier, Vattikuti, Purcell and Lee2015). SambaR performs diverse clustering methods to analyse SNP data: Principal Component Analysis (PCA), Discriminant Analysis (DA), and Bayesian clustering. To run the analyses, we set a maximum of missing data per individual of 25% (indmiss = 0.25) and per SNP of 10% (snpmiss = 0.1). We also performed Bayesian clustering algorithms in STRUCTURE (Pritchard et al. Reference Pritchard, Stephens and Donnelly2000) using the admixture ancestry model and correlated allele frequencies. Markov Chain Monte Carlo (MCMC) models were fixed at 750,000 iterations, discarding the initial 250,000 as burn in, and K varying from 1 to 3 (conducting 10 replicates per K value with a different random seed). We used structure harvester v0.6.94 (Earl and von Holdt Reference Earl and von Holdt2012) and clumpp v1.1.2 (Jakobsson and Rosenberg Reference Jakobsson and Rosenberg2007) to combine results from replicate runs and calculate the average membership coefficients of each individual to each cluster.
Results
MtDNA sequences of the 71 Hooded Grebe individuals showed seven variable sites defining 11 haplotypes (GenBank Accession Numbers OR760039–OR760049). Two haplotypes were frequent (H1, H3), four were less frequent (H2, H5, H9, H10), and five were rare (Figure 1A). Diversity values for the entire population were h = 0.77 and π = 0.003. Pairwise ΦSTs were low and only significantly different between the southernmost SIB and the northernmost BAP (SIB-BAP ΦST= 0,09, P = 0,03). ST was not significantly different from either of the other two plateaus (ST-BAP ΦST= 0,00, P = 0,75; ST-SIB ΦST= 0,06, P = 0,06; Figure 1).
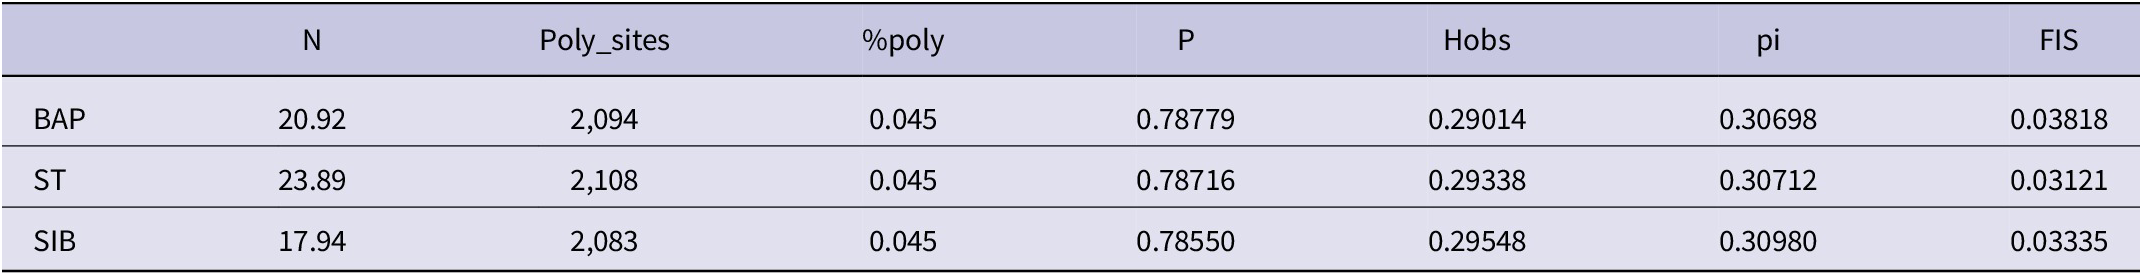
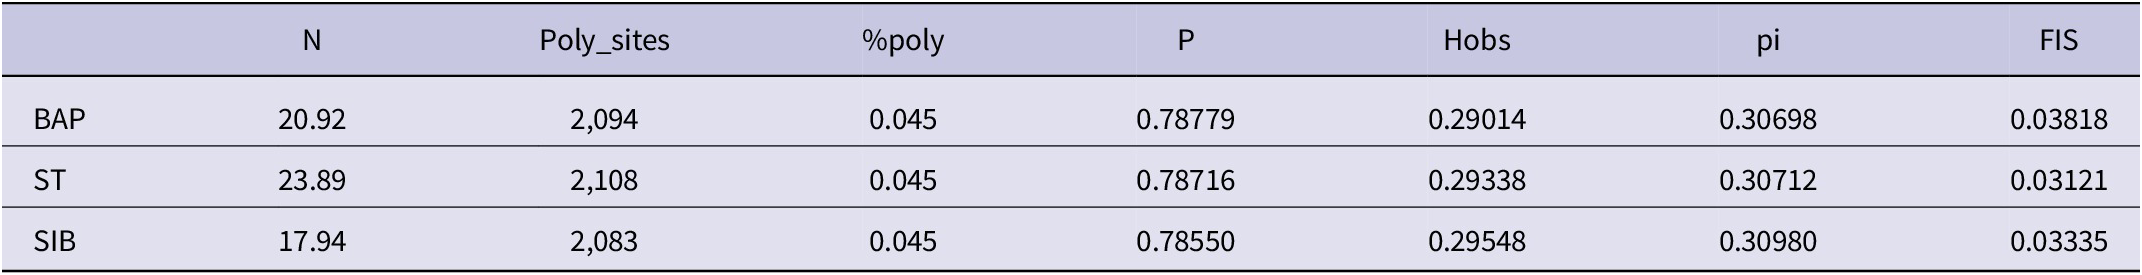
We recovered a total of 2,120 SNPs in 1,886 RAD loci across 63 individuals after completing all filtering processes. Diversity values were similar among populations (Table 1). Pairwise differentiation among populations was not significant (P >0.5). The average FST value between pairs of populations was FST= 0.01 (0.0137–0.0157) and consistently low among all SNPs.
Summary genetic statistics across 2,120 variable RAD sites for the three populations (BAP = Lake Buenos Aires Plateau, ST = Strobel Plateau, SIB = La Siberia Plateau). These statistics include the average number of individuals genotyped at each locus (N), the number of polymorphic nucleotide sites across the data set (Poly_sites), percentage of polymorphic loci (%poly), the average frequency of the major allele (P), the average observed heterozygosity per locus (Hobs), the average nucleotide diversity (pi), and the average Wright’s inbreeding coefficient (FIS)
Different analyses for population structure showed consistent results grouping all individuals in one cluster, independently of the plateau of origin. The proportion of missing data was low for individuals (mean = 0.02) and for SNPs, of which 148 were discarded. PCA based on 1,738 retained SNPs did not separate individuals by plateaus but grouped them in one cluster with only a few individuals from different plateaus showing some genetic distance from the majority (Figure 1B). Bayesian clustering algorithms also showed the highest log-likelihood for one cluster (K = 1). Clustering in three groups (K = 3) did not assign individuals to plateaus (Figure 1C). Finally, the DA including three clusters also assigned almost all individuals to the same group (Figure 1D).
Discussion
We did not find differences between plateaus in population structure of Hooded Grebes. Nuclear markers did not separate individuals by plateaus but pooled them into one cluster containing all individuals belonging to three different reproductive populations. For mtDNA, we found a low differentiation between individuals belonging to the northernmost and southernmost plateaus included in the study, BAP and SIB, respectively. Thus, genetic markers do not show the pattern of differentiation expected for a long-lasting and strict philopatric behaviour towards the breeding plateaus. Our results, stemming from c.10% of the global population, also show that genetic diversity indices are within the range of the mean values found in birds (Ellegren Reference Ellegren2013), indicating that no significant loss of genetic variability has yet occurred, despite the dramatic population decline the species has suffered in the last years. Since the reduction in population size occurred between the 1980s and early 2000s and the generation time is supposed to be relatively long (Fjeldså Reference Fjeldså1986), it is possible that individuals still retain ancestral genetic variability.
The hypothesis of site fidelity was based mostly on field observation. For 10 consecutive breeding seasons (2012–2022), approximately the same number of individuals was observed at different plateaus (Roesler et al. Reference Roesler, Lancelotti, Gabarain, Buchanan, Hernández, Fasola and Schulenberg2025). A plausible explanation for the absence of a genetic pattern despite observational evidence is that Hooded Grebes exhibit reproductive but not natal philopatry. In this scenario, after the first migration towards the estuaries, first-year individuals return to any of the plateaus without selecting the one where they were raised, returning to that last plateau during the following reproductive attempts. In this scenario, a genetic differentiation among plateaus is not expected.
Differences between natal and reproductive philopatry might be related to the strength of parent–offspring associations. It has been shown that migratory behaviour has a genetic basis (Berthold and Querner Reference Berthold and Querner1981; Helbig Reference Helbig1991; Merlin and Liedvogel Reference Merlin and Liedvogel2019), but is also culturally transmitted in many species, where the bond between parental individuals and their offspring determines the first migration of juveniles (Sutherland Reference Sutherland1998). Roesler et al. (Reference Roesler, Lancelotti, Gabarain, Buchanan, Hernández, Fasola and Schulenberg2025) mentioned an association between adults and juveniles in autumn migration, but not a strict association, since some juveniles remain at different wintering grounds than the adults. In European grebes, it has been found that fidelity to the breeding site is more pronounced in adult individuals than in juveniles, suggesting that natal philopatry might not be as strong as reproductive philopatry (Konter and Konter Reference Konter and Konter2006), with breeding dispersal being less pronounced than natal dispersal (Paradis et al. Reference Paradis, Baillie, Sutherland and Gregory1998).
A second explanation is that Hooded Grebe has both natal and reproductive philopatric behaviour, but that this behaviour is not fixed. A relaxed philopatry, with eventual movements between lakes and/or plateaus, might arise from unstable conditions of certain lakes/plateaus. This kind of dispersion between nearby lakes within the same plateaus was mentioned in the past when the conditions in a year were unfavourable (Lange Reference Lange1981). The same situation was also detected between plateaus, when lakes dry up completely, as is the case of Cerro Ventana Plateau in 2010, where the populations disappeared (Roesler Reference Roesler2016). Although the fate of Cerro Ventana’s individuals is unknown, it could be linked to dispersal or, alternatively, simply to populations becoming locally extinct.
Migration and movement features can change with global warming. Visser et al. (Reference Visser, Perdeck, Van Balen and Both2009) showed that global warming induced declines in migration distance in many bird species in north-west Europe. Climate change may thus not only result in strong shifts in phenology and species breeding ranges (Parmesan and Yohe Reference Parmesan and Yohe2003; Root et al. Reference Root, Price, Hall, Schneider, Rosenzweig and Pounds2003; Visser and Both Reference Visser and Both2005), but also in changes in migration timing, passage, and wintering areas, and consequently the entire annual cycle of migratory birds (Berthold Reference Berthold2001). A thorough study on Hooded Grebes’ habitat availability at ST (Lancelotti et al. Reference Lancelotti, Pessacg, Roesler and Pascual2020) showed a marked reduction of lakes during the last four decades due to climatic changes. Banding information suggests that during dry periods, like 2022–2023 (IR), the proportion of marked individuals relocated outside their “plateaus of origin” increases (i.e. individuals banded in one plateau and reobserved in a different one; Roesler et al. Reference Roesler, Lancelotti, Gabarain, Buchanan, Hernández, Fasola and Schulenberg2025). Banded individuals from SIB were found in ST, and individuals from BAP were also found in ST. However, no individuals banded in BAP or in SIB were found south or north of ST, respectively (Roesler et al. Reference Roesler, Lancelotti, Gabarain, Buchanan, Hernández, Fasola and Schulenberg2025). These findings relate to the mtDNA differences found between individuals of the more distant plateaus. This might well fit with the pattern suggested above, that under unfavourable lake/plateau conditions, individuals disperse but within close areas, not dispersing randomly to any of the other plateaus. Therefore, a “relaxed” philopatry, conditioned by external conditions might be operating in Hooded Grebes.
A slight differentiation between the northernmost (BAP) and the southernmost (SIB) plateaus in mtDNA, but not nuclear DNA, might be related to dispersal differences between sexes (Prugnolle and de Meeus Reference Prugnolle and De Meeus2002). There is no information on sex-biased dispersal in grebes. A relevant implication of the existence of this different rate of dispersal between sexes is that conservation efforts might focus on supplementing depressed populations with females since males have higher chances of colonisation.
The identification of management units or conservation units (Moritz Reference Moritz1994; Palsbøll et al. Reference Palsbøll, Berube and Allendorf2007) is essential to maintain the adaptive potential of threatened species and address appropriate conservation and management strategies (Allendorf and Luikart Reference Allendorf and Luikart2007; Fraser and Bernatchez Reference Fraser and Bernatchez2001). We were unable to identify management units for the Hooded Grebe. The genetic patterns we observed do not support a strict philopatric behaviour towards reproductive plateaus. On the contrary, our results suggest that the Hooded Grebe is adapted to a variable, rather than a stable, environment, requiring large areas where individuals can search for proper breeding habitats during different climate conditions. Evidence shows that migratory traditions are not static and that migration routes, stop-over sites, and migration phenology are dynamic systems evolving over time (Jonker et al. Reference Jonker, Kraus, Zhang, van Hooft, Larsson and van der Jeugd2013). A philopatric behaviour intended to maximise fitness outcomes is probably an interplay of fixed and plastic movements that optimise the use of known habitats but also allows flexible responses to varying environments (Clausen et al. Reference Clausen, Madsen, Cottaar, Kuijken and Verscheure2018). The plasticity of some birds where individuals switch between strategies in response to previous experience, suggests that those individuals explore environmental conditions to adopt an optimal migration strategy (Madsen Reference Madsen2001). These changes can be magnified manifold by the influence of these individuals on conspecifics copying their choice. Such cultural transmission between individuals is probably a common phenomenon among migrating social birds (Jonker et al. Reference Jonker, Kraus, Zhang, van Hooft, Larsson and van der Jeugd2013; Mueller et al. Reference Mueller, O’Hara, Converse, Urbanek and Fagan2013). Thus, Hooded Grebes might have responded to environmental changes in the past, as well as the present, moving towards suitable breeding and wintering sites, showing only a recent use of the plateaus in evolutionary terms and a current switch of plateaus due to unfavourable conditions. Further studies on marked individuals will give us more information about natal and reproductive philopatry and the tendency for individuals to return to their reproductive plateaus depending on sex.
Relevant actions to protect the species need to switch from strategies focused on conserving spatially limited restricted areas (i.e. only focused on nature reserve creation) to collaborative, large-scale, mixed land-management strategies. These should include the creation of protected areas, as well as the restoration and protection of private lakes (i.e. collaborative work with fish farmers and sport fishermen). Moreover, our results are highly relevant for a current programme that actively recovers ecologically lost eggs from the wild to produce juveniles by hand rearing to reinforce and maximise annual population recruitment (Gabarain et al. in prep.). The lack of genetic structure allows us to use those individuals to reinforce all plateaus’ populations, regardless of their origin. This is especially important since there has been a strong reduction in some of those plateaus with almost no reproduction in over a decade (Roesler et al. Reference Roesler, Lancelotti, Gabarain, Buchanan, Hernández, Fasola and Schulenberg2025).
Acknowledgements
Fieldwork was conducted thanks to the support of donors to Hooded Grebe Foundation and Aves Argentinas, especially International Conservation Fund of Canada (ICFC), Whitley Fund For Nature, the Preventing Extinction Programme of BirdLife International (Ben Olewine and Britt and Steve Thall), EDGE of Existence Programme (Zoological Society of London), CREOI, Toyota MC (Argentina and International), Nippon Car, among others. We have essential support from the Environmental Secretary of Santa Cruz (Lic. Marino Bertinat) and ranch owners (Tonchi and Maria, Angel Rodríguez, Pedro and Juan Garitaonandia, Flia. Hormachea, Torcuato Sozio, Alberto Alba, Julian Escalada and Charly Cassanello -Jurassik Lodge- and many others) and the puesteros (Nazareno, Pancho Chicahuala, Segundo Jara, Pescado Ruíz, Alcides Castro, and many others). We thank Susan Mbedi and Sarah Sparmann for their support in library preparation and sequencing. Ignacio Roesler, Laura Fasola, Julio L. Lancelotti, Juan C. Reboreda and Bettina Mahler are researchers at CONICET. Gabriela Gabarain is Phd fellow at CONICET. Part of the research was financed by PICT 2016-2646 (CONICET).
Supplementary material
The supplementary material for this article can be found at http://doi.org/10.1017/S0959270925100142.