Introduction
Maternal undernutrition, small size at birth, preterm birth and accelerated growth in early childhood, which often follows reduced size at birth and preterm birth, are all associated with increased risk for obesity and metabolic diseases later in life.Reference Newsome, Shiell and Fall1–Reference Jaquiery, Oliver, Honeyfield-Ross, Harding and Bloomfield7 This increased predisposition to adult disease following early life events that may be amplified by postnatal factors such as lifestyle and diet.Reference Vickers, Breier, McCarthy and Gluckman8 We have recently demonstrated that periconceptional maternal undernutrition in sheep impairs glucose tolerance and hypothalamic–pituitary–adrenal axis function in adult offspring and leads to increased adiposity in adult males.Reference Jaquiery, Oliver, Honeyfield-Ross, Harding and Bloomfield7, Reference Todd, Oliver, Jaquiery, Bloomfield and Harding9, Reference Oliver, Bloomfield and Jaquiery10 Recent data indicate that lifestyle behaviour may also be influenced by prenatal and early life environmental exposures: weReference Begum, Stevens and Smith11 and othersReference Taylor and Poston12 have shown that maternal undernutrition alters offspring neuronal appetite regulatory circuits, potentially leading to increased appetite and/or decreased satiety signals. The other behavioural component of the energy balance equation is energy expenditure, and decreased physical activity/sedentary behaviour combined with altered appetite regulation could have profound effects on obesity and metabolic syndrome susceptibility. Maternal undernutrition throughout pregnancy in rats leads to decreased physical activity in pre-pubertal and adult offspringReference Vickers, Breier, McCarthy and Gluckman8; however, there are no data on the effects of undernutrition confined to the period around conception on physical activity of the offspring. We hypothesized that maternal undernutrition in sheep only in the periconceptional period would result in decreased voluntary physical activity in adult offspring.
Methods
Ethics approval for this study was obtained from the University of Auckland Animal Ethics Committee. The nutritional paradigm has been described previously.Reference Oliver, Bloomfield and Jaquiery10 Briefly, 4- to 5-year-old Romney ewes were undernourished from 61 days before conception to day 30 of gestation (UN), with nutrition individually adjusted to achieve a 10–15% weight loss. By mating, intake of UN ewes was 80% of controls (CON). Ewes were lambed naturally and there was no difference in the birth weight between groups.Reference Oliver, Bloomfield and Jaquiery10 Lambs were weaned at 3 months of age and kept on pasture with a flock of same-sex peers, as is standard farming practice in New Zealand, except when weighed or brought indoors for specific investigations as reported elsewhere.Reference Todd, Oliver, Jaquiery, Bloomfield and Harding9, Reference Hernandez, Harding and Oliver13, Reference Hernandez, Matthews, Oliver, Bloomfield and Harding14
To measure spontaneous locomotor activity in the form of total distance travelled in the paddock under normal grazing conditions, 18-month-old offspring were moved in batches of four to a 0.75 ha (7500 sq m) rectangular dedicated paddock, where they were left undisturbed during the 48 h observation period. Ewes’ oestrous cycles were synchronized using intravaginal progesterone releasing devices at least 4 days before the tests to avoid the confounding effects of the oestrous cycle on the behaviour of the ewes. A GPS Lassen iQ module (Trimble Navigation Limited, Sunnyvale, CA, USA) enclosed in a small plastic case (55 × 40 × 85 mm) to protect it from the environment was secured to the back of each animal using a ram-harness. At the end of the 48 h period, the equipment was removed and the data were downloaded. As the coordinates retrieved from the GPS were recorded as ‘world geodetic system’ coordinates, we converted them to New Zealand Map Grid coordinates using the Concord2 coordinate conversion programme (Copyright 2011 Crown copyright, Land Information New Zealand and the New Zealand Government). The New Zealand Map Grid coordinates were then processed using the geographic information system ArcGIS Programme (Esri, New York). We used GPS monitoring because it was the least intrusive method available at the time the measurements were taken, could be attached to the animals’ backs with low risk of dislodgement and reliably measures distance travelled and not limb movement, such as step counters, which provide less reliable data.
Measurements taken while moving the sheep into and out of the paddock were excluded, and data were analysed for erroneous GPS measures. The 48-h period was divided into daylight and non-daylight hours for the farm location, and the percentage of total hours in daylight calculated to adjust for any effects of daylight and time of year that the experiments were conducted. The average time between GPS measurements (ATBGM) was also calculated for each animal, as weather patterns may affect the time between locations computed from satellite tracking of the GPS modules and because sheep do not move in a straight line from one location to another, meaning that two points separated by a greater time interval may underestimate the actual distance travelled. There was a significant inverse relationship between the ATBGM and the distance travelled. Animals for which average time between data points fell outside 1.5 times the interquartile range were excluded.
Data were assessed for normality and analysed using multiple linear regression modelling. Explanatory variables included sex, nutrition group, singleton/twin status, ATBGM, percentage of total hours in daylight, batch effect for animals that were monitored in the paddock at the same time and an interaction term for sex and nutrition. Ewe identity was entered as a random effect to account for non-independence of twins within pairs. Data are expressed as mean or least square means with s.e.
Results
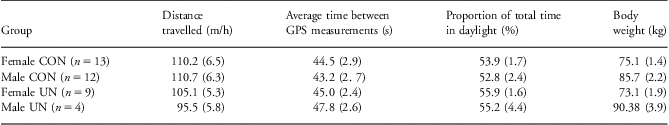
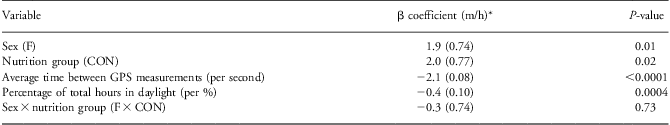
A total of 38 animals (12 singletons and 26 twins) were included in the analysis (female CON, n = 14; male CON, n = 12; female UN, n = 8; male UN, n = 4). There were no significant differences between groups for ATBGM or for percentage of daylight hours (Table 1). All groups contained both twins and singles (female CON 11 twins and four singles, male CON nine twins and three singles, female UN six twins and three singles, and male UN two twins and two singles). There was no effect of twin conception or test batch, and absolute body weight was not significantly different between nutritional groups (Table 1). Mean distance travelled per hour [unadjusted group means (s.e.)] was greater for CON than UN animals [110.4 (4.4) v. 101.9 (4.1) m/h], and greater for females than males [108.4 (4.5) v. 106.9 (5.1) m/h] (Table 1). Significant effects (Table 2) were observed for sex [least squared means (s.e.): female, 108.6 (0.9); male, 104.7 (1.2); P = 0.01] and nutrition group [CON, 108.6 (0.3); UN 104.7 (1.3) m/h; P = 0.02], but not for the sex by nutrition group interaction (P = 0.73), indicating that the direction of the effects between groups did not differ by sex. The adjusted r 2 for the model was 0.98.
Distance travelled, time between GPS measurements, daylight hours and adult body weight in offspring of undernourished ewes and controls
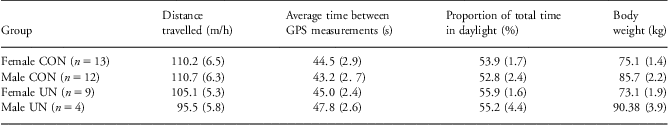
Data are mean (s.e.).
Multiple regression analysis for average distance travelled
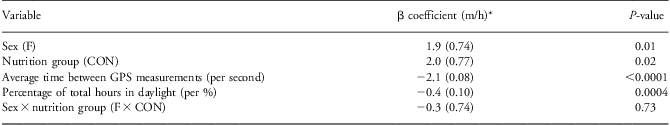
*Data are mean (s.e.). Overall model adjusted r 2 = 0.98.
Discussion
We have shown that maternal undernutrition from 61 days before conception to day 30 of gestation led to decreased voluntary activity in the form of total distance travelled under normal paddock grazing conditions in adult offspring. There is a growing body of data demonstrating that maternal undernutrition during pregnancy can adversely affect offspring metabolic health and obesity later in life; however, few studies have examined how the intrauterine environment can affect voluntary activity in adulthood. Vickers et al. Reference Vickers, Breier, McCarthy and Gluckman8 showed in rats that a substantial maternal nutritional restriction (30% of CON) maintained throughout pregnancy leads to decreased physical activity and hyperphagia in adult offspring, effects that are exacerbated by postnatal overnutrition (hypercaloric diet with 30% fat) but ameliorated by neonatal leptin treatment.Reference Vickers, Gluckman and Coveny15 Our data are consistent with these findings but show that a moderate maternal undernutrition lasting only for the first 30 days of a 150-day pregnancy, followed by ad libitum intake resulting in a restoration of maternal body weight and not affecting offspring birth weight, is sufficient to permanently alter voluntary activity of the adult offspring. Our data are also unique because we measured voluntary activity of a large domesticated mammal in its natural environment.
If these data translate to the human setting, this would mean that alterations in maternal diet once pregnancy is confirmed would likely be too late to prevent these effects. It is also important to note that there were no differences in birth weight between UN and CON animals in this study; thus, the outcomes are not related to small size at birth or accelerated postnatal growth. Rather, the brief nutritional insult around conception appears to have resulted in a variety of adaptations leading to a propensity to obesity and an adverse metabolic phenotype in adulthood, including in appetite regulatory pathways, the glucose–insulin and HPA axes.Reference Todd, Oliver, Jaquiery, Bloomfield and Harding9–Reference Begum, Stevens and Smith11 Because the animals in our study were free living in the paddock, we were unable to measure food intake directly. However, it seems likely that an underlying mechanism for these effects is epigenetic programming of genes regulating feeding and activity behaviour, and therefore energy intake and expenditure in the ventral hypothalamus. We have previously demonstrated that the periconceptional undernutrition paradigm described in this study results in altered methylation and histone acetylation of the glucocorticoid receptor (GR) and proopiomelanocortin promoter regions in the ventral hypothalamus in both singletons and twins consistent with increased expression of GR in the appetite regulatory centres of the brain.Reference Begum, Stevens and Smith11, Reference Stevens, Begum and Cook16 GR is known to be involved in the regulation of the orexigenic and anorexigenic hormones of the hypothalamus and these changes may therefore have an impact on the appetite/energy expenditure balance in postnatal life. Indeed, we have recently demonstrated that the changes in GR do persist through to adulthood (5 year), with increased GR mRNA and protein expression and altered expression of appetite regulatory genes (unpublished data).
Our data also demonstrate a sexually dimorphic response, with male offspring from periconceptionally undernourished mothers being ∼14% less active than males from CON mothers, whereas female offspring from undernourished mothers were only 2% less active than females from CON mothers. Without knowing resting metabolic rates of these animals and the caloric expenditure resulting from the recorded distances travelled, it is difficult to determine the associated differences in total energy expenditure. There are few data reporting how undernutrition during pregnancy affects metabolic rateReference Sandboge, Moltchanova and Blomstedt17, Reference Gardner and Rhodes18; however, over time, a 14% difference in voluntary daily activity is likely to lead to a substantial difference in total energy expenditure and subsequent weight gain if there is no concurrent decrease in energy intake. Further, it has been hypothesized that intrauterine exposure to undernutrition causes male offspring to direct resources towards energy conservation and reproduction, with resulting susceptibility to obesity if the offspring is then born into an environment where nutrition is not limited.Reference Gluckman, Hanson, Spencer and Bateson19 Our finding of a greater reduction in distance travelled by males in this study is consistent with this hypothesized reduction in energy expenditure, and we have previously reported increased testis size in male offspring,Reference Jaquiery, Oliver, Honeyfield-Ross, Harding and Bloomfield7 consistent with the hypothesized greater resource allocation to reproduction. Conversely, females from undernourished mothers have smaller ovaries.
A potential limitation of this study is that we do not have measures of fat mass in the animals at the time of this study, and therefore we cannot draw causal inferences about the relationship between voluntary activity and obesity. Fat mass was measured by dual energy X-ray absorptiometry at 5 years of age, by which time male offspring of undernourished ewes had significantly greater fat mass.Reference Jaquiery, Oliver, Honeyfield-Ross, Harding and Bloomfield7 It is possible that reduced activity led to later increased fat mass or, alternatively, that the offspring of undernourished ewes already had a different body composition with a higher percentage of body fat and lesser lean mass at the time of study, thereby having similar body weight, and this led to reduced activity. However, absolute body weight was not significantly different between nutritional groups, suggesting that an effect on activity is unlikely. Decreased activity predisposing to obesity would be consistent with the data by Vickers et al.,Reference Vickers, Breier, McCarthy and Gluckman8 who reported reduced voluntary activity in rats at 35, 145 and 420 days of age in offspring from dams that were undernourished throughout pregnancy, with decreased activity preceding onset of obesity.
In summary, these data demonstrate that maternal undernutrition around the time of conception significantly decreases voluntary activity in 18-month-old sheep, particularly in males, despite restoration of sufficient nutrition from ∼20% of gestation. It remains to be determined whether poor maternal nutrition in women before or around the time of conception may have similar effects, potentially predisposing offspring to an increased risk of obesity and metabolic disease in later life.
Acknowledgements
None.
Financial Support
This work was supported by Health Research Council grant # 05/193, Dr. Frank Bloomfield and Gravida: National Research Centre for Growth and Development grant # NRCGD 06021JH, Dr. Frank Bloomfield.
Conflicts of Interest
None.
Ethical Standards
The authors assert that all procedures contributing to this work comply with the ethical standards of New Zealand and the University of Auckland and with the Helsinki Declaration of 1975, as revised in 2008, and has been approved by the institutional committees, University of Auckland Animal Ethics Committee. The authors assert that all procedures contributing to this work comply with the ethical standards of the New Zealand and University of Auckland guides on the care and use of laboratory animals, and this work has been approved by the University of Auckland Animal Ethics Committee.