Introduction
Starch in cereals is important to newly weaned piglets since by weight it constitutes the largest portion of the diet and is the major energy-yielding component. The rate of starch digestion is therefore a crucial characteristic that governs the dietary energy value of compound diets (Wiseman, Reference Wiseman2006). Cereals, and in particular wheat, have generally been considered to be of comparatively constant nutritional value, regardless of their variety, endosperm texture and growing environment. However, considerable variations in starch digestibility between cereals, and also among varieties within the same species, have been reported (Short et al., Reference Short, Gilbert, Wiseman, Boorman, Snape, Orford, Angus and Wakeman1998; Weurding et al., Reference Weurding, Veldman, Veen, van der Aar and Versegen2001). Currently, no firm explanations for these large variations are available, although they may be caused by a number of factors, such as genetic variability between and within cereal species (Wiseman, Reference Wiseman2000; Rudi et al., Reference Rudi, Uhlen, Harstad and Munck2006), content and nature of non-starch polysaccharides (Holtekjølen et al., Reference Holtekjølen, Uhlen, Bråthen, Sahlstrøm and Knutsen2006) and, mainly in the case of wheat, endosperm texture (Wiseman, Reference Wiseman2000). Reliance on variety name in the design of nutrition studies is not robust, as two varieties may be closely or distantly related. Name alone would give no guide as to their genetic relationship (Wiseman, Reference Wiseman2000). It is for this reason that, for wheat, a new approach based on assessing near-isogenic lines (two lines of similar background differing essentially in only one key characteristic) was developed. Through this, the negative effects of the 1B/1R rye translocation, where the short arm of the chromosome 1B of wheat has been replaced with the short arm of the 1R chromosome of rye, and of hard endosperm texture (although the two factors may interact) have been established (Short et al., Reference Short, Wiseman and Boorman2000).
To date, analysis of raw cereals in animal trials has generally been limited to determination of their gross chemical composition by proximate analysis. However, these measurements provide no useful information on the physical behaviour of the diets or the properties of dietary starch in relation to its digestibility. A number of recent reviews have tentatively identified the structural features of starch that may potentially have marked effects on its digestibility (Svihus et al., Reference Svihus, Uhlen and Harstad2005; Stevnebø et al., Reference Stevnebø, Sahlstrøm and Svihus2006; Tester et al., Reference Tester, Qi and Karkalas2006). For cereal-based feeds, key characteristics that can affect digestibility are likely to be associated with the matrix in which the starch is embedded. The hydration properties, surface area, solubility of the materials and the ability to mix with enzymes and digestive juices may have a major influence on the digestive break down and general behaviour within the gastrointestinal tract. A recent review (Doucet et al., Reference Doucet, White, Wiseman and Hill2007) has highlighted a number of parameters that are typically used to screen cereals in human foods that could be adopted for monitoring animal feeds. Some of these parameters include nutritional features of the materials, while others act as a general fingerprint for the raw or cooked feed. These measures fall into three categories: (i) hydration characteristics, (ii) structural properties and (iii) in vitro amylolytic digestion. Using these measures, good correlations between in vitro data for raw and extruded wheats and the corresponding in vivo data of starch digestibility have been demonstrated in the newly weaned piglet (Doucet et al., Reference Doucet, White, Wiseman and Hill2007). This indicated that in vitro assessment could provide additional information that can contribute to a more complete understanding of digestibility.
The current study, for the first time, relates the measured physicochemical properties of eight raw cereals to the biological responses of newly weaned piglets. The objectives of the trials were to confirm whether the measured physicochemical properties of starch from (i) hard and soft endosperm wheat cultivars (trial 1) and (ii) seven cereals (trials 2 and 3) relate to in vivo starch digestibility and to changes in the gut environment of newly weaned piglets.
Material and methods
Piglet trials
Animals, housing and management
Entire male piglets (Large White × Landrace; 8 to 12 kg live weight) were obtained immediately on weaning at 28 days of age. Animals (trial 1: n = 22, trials 2 and 3: n = 44) were individually weighed, transferred to an environmentally controlled (28°C to 32°C; 16L:8D lighting regime) experimental unit, housed in individual pens with semi-slatted floors, two nipple drinkers and a feed trough. The piglets were randomly allocated to a specific experimental diet, which was fed in meal form and on an ad libitum basis. Fresh water was also available ad libitum. The experimental period was 14 days. Pigs used in trial 3 shared the same genotype, but were sourced from a different supplier from those animals in trials 1 and 2. Experimental procedures were conducted under the official code of practice and ethical procedures relating to animal trials at Nottingham.
Diets
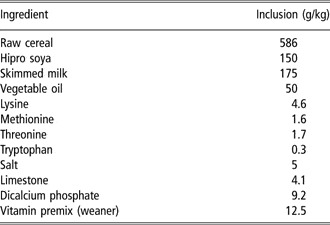
Nine experimental diets were evaluated, each containing a source of raw starch, in the form of cereals, incorporated at the same rate of 586 g/kg (Table 1). Diets did not contain antibiotic growth promoters or zinc oxide. A total of eight cereals, with a wide range of physicochemical properties, were selected for nutritional evaluation. The cereals were ground through a 1.5-mm screen using a hammer mill and mixed with the basal diet. Diets were manufactured in the University of Nottingham experimental animal feed mill.
Diet specification (experimental diets) in trials 1, 2 and 3

Trial 1
Two near-isogenic wheat samples (Hard (HW) and Soft (SW); with endosperm hardness of 11.2 and 6.3, respectively, as measured with the Bran & Luebbe Infra-analyser 260 NIR with a built-in calibration; data approximate to two times the Stenvert hardness scale on which 4 to >7 is ‘hard’ milling and 1 to 3 is ‘soft’) were supplied by Nickersons (UK) Ltd (Market Rasen, Lincolnshire, UK) as a single batch grown under the same agronomic conditions at the same location. Two assumed iso-energetic (14.4 MJ digestible energy (DE)/kg) and iso-nitrogenous (235 g crude protein (CP)/kg) experimental diets (D HW and D SW) were formulated. Two piglets (Control) were slaughtered on day 0, with two piglets from each dietary group slaughtered at days 2, 4, 6, 10 and 14 post weaning (n = 4 on each day, two per diet).
Trials 2 and 3
Four experimental diets were evaluated in each trial. Diets used in trial 2 contained either soft wheat (control; D W1), barley (D B), rye (D R) or triticale (D T), while those used in trial 3 were composed of either soft wheat (control; D W1), maize (D M), whole oats (D WO) or naked oats (D NO). For these two trials, four piglets (Control) were slaughtered on day 0, with two piglets from each dietary group slaughtered at days 2, 4, 6, 10 and 14 post weaning (n = 8 on each day, two per diet). The soft wheat used in trial 1 and in trials 2/3 was of the same variety, grown by the same breeder at the same site but on 2 consecutive years.
Statistical model
Data were subjected to analysis of variance (ANOVA) using a fully randomised design (Genstat v. 8.1, 2005; Lawes Agricultural Trust, Rothamsted, UK) with dietary cereal as the main factor. For the gut morphology measurements, piglet live weight was employed as a covariate in the statistical analysis.
In vivo analysis
At slaughter, the small intestine was removed and sections of 6 to 8 cm in length were cut at distances of, proportionately, 0.25, 0.5 and 0.75 along the gastric pylorus to the ileocaecal valve. Details of how gut sections were treated are provided in Zarkadas and Wiseman (Reference Zarkadas and Wiseman2005). Slides were stained using the trichrome procedure and measurements of villus height (VH), villus width (VW) and crypt depth (CD) were taken for each pig (n = 10 per section). VH-to-CD ratio (VH : CD) was recorded for each pig. Gut morphology sections were observed and measured using video frame grabber (Model Flashpoint 3d Lite; Integral Technologies Inc., rue Berlier. Laval, Canada) and Scion Image for windows (v. Beta 4.02; Scion Corporation, Frederick, MD, USA).
Digesta from individual pigs were taken at slaughter from 0.25, 0.5 and 0.75 along the small intestine. Fresh digesta samples (1.5 ml) were centrifuged (9000 × g for 6 min) and supernatant viscosity (0.5 ml) was determined using a Brookfield DV-III and cone plate rotational viscometer (CP40; Brookfield Engineering Laboratories, Middleboro, MA, USA) attached to a water bath at a temperature of 39.6°C. Digesta not used for determining viscosity were stored at −20°C for subsequent laboratory analysis. A lack of sufficient digesta at the 0.25 site in many of the pigs meant that determination of starch and nitrogen at this region could not be performed.
Chemical analysis of diets, digesta and faecal samples
All analyses were conducted in duplicate with repetition if variation was >5%. Diet samples were dried for approximately 48 h in a forced draft oven set at a temperature of 105°C for dry matter (DM). Digesta and faecal samples were freeze-dried prior to laboratory analysis. Caecal digesta samples were frozen (−80°C) until needed for analysis. The nitrogen (N) content was determined using an NA 2000 Nitrogen Analyser (Fisons Scientific Equipment, Loughborough, UK). Starch content was estimated by solubilisation of starch with dimethyl sulphoxide, sodium acetate buffer and amyloglucosidase enzyme solution using a total starch assay kit (Megazyme, Wicklow, Ireland; AOAC method 996.11, AACC method 76.13). A GOPOD glucose determination reagent solution was used to quantify the released glucose by reading the absorbance with a SP6-500 UV spectrophotometer (Pye Unicam Ltd, Cambridge, UK) at 510 nm.
Calculation of results
Individual daily feed intake (FI) was recorded for all piglets. Total FI was divided by the number of days that the animal took to grow over the specific live weight range of the experiment giving average daily FI. Chemical analysis of diets, digesta and faeces (including acid-insoluble ash as an inert marker) allowed the calculations of coefficient of total tract apparent digestibility (CTTAD) and coefficient of ileal apparent digestibility (CIAD) of nitrogen and starch.
Determination of caecal volatile fatty acids (VFA)
VFA analysis of caecal digesta was performed using gas liquid chromatography based on the method of Franklin et al. (Reference Franklin, Matthew, Vickers and Clift2002). Molar proportions of each of the individual acids were then calculated by dividing sample concentrations obtained for each acid by the total concentration of all six VFAs.
In vitro feed characterisation
Samples
For trial 1, the milling characteristics of hard and soft wheats were studied by analysing whole milled samples. Sieved fractions (212 to 250 μm) from the milled samples were used in the characterisation tests. This was to reduce differences arising from having different particle sizes due to the disparities in milling behaviour. For trials 2 and 3, cereal flours without further size fractionation were analysed. Experimental diets used in all three trials were also analysed. The moisture content of cereal samples and diets was determined by oven drying at 105°C for 18 h and calculated as an average value of triplicates.
Hydration properties
Pasting of cereal flours and diets was analysed using a Rapid Visco Analyser Series 4 (RVA; Newport Scientific, Warriewood, NSW, Australia), along with the accompanying software Thermocline for windows v. 2.0 (Newport Scientific). The RVA allows precise and reliable measurements of the viscosity of materials while being sheared under defined hydration and temperature regimes. A difference in any RVA parameter between samples that is greater than 5% is considered to be significant (P < 0.05; Becker et al., Reference Becker, Hill and Mitchell2001). The RVA provides a number of pasting parameters (e.g. cold swelling peak, gelatinisation peak, trough and final viscosity), which represent a relative measure of starch gelatinisation, disintegration, swelling and gelling ability (Ruy et al., Reference Ruy, Neumann and Walker1993; Ravi et al., Reference Ravi, Sai Manohar and Haridas Rao1999). RVA measurements were performed using 3 g of cereal flour (dry weight) and 25 g of distilled water, whereas 5.17 g of diet sample (dry weight) was used to compensate for the amount of starch. Sample and water were weighed separately to ±0.001 g, mixed and measurements started within 20 s. The pasting profile used started at 25°C and was held for 10 min, ramped to 95°C over 6.5 min, held at 95°C for 6.5 min, cooled back to 25°C over 10 min, and finally held at 25°C for 7 min. Each analysis took 40 min and was performed in duplicate.
The RVA pasting profile was also used to assess the presence of endogenous amylase in cereals (Noda et al., Reference Noda, Ichinose, Takigawa, Matsuura-Endo, Abe, Saito, Hashimoto and Yamauchi2003), by pasting cereal flours in 25 g of silver nitrate (AgNO3; 0.5 mmol/dm3) instead of 25 g of distilled water. AgNO3 is an effective endogenous amylase inhibitor and a concentration of 0.5 mmol/dm3 was sufficient to fully inhibit α-amylase activity for all tested cereals. Amylase activity was estimated by calculating the ratio [(PVAg − PVH2O)/PVH2O], where (PVAg) is the RVA pasting parameter of peak viscosity determined in AgNO3, and (PVH2O) is that determined in water. This ratio was found to be positively correlated (0.96) to α-amylase activity (Noda et al., Reference Noda, Ichinose, Takigawa, Matsuura-Endo, Abe, Saito, Hashimoto and Yamauchi2003).
Water absorption (WAI) and water solubility (WSI) Indices of cereal flours were also determined. These are two quantifiable parameters that assess the swelling and solubility behaviour of the starch component of cereals in excess water. WAI represents the volume occupied by the hydrated starch following swelling in excess water, whereas WSI denotes the amount of soluble polysaccharides released from the granules to the aqueous phase. WAI and WSI were determined by mixing 0.3 g of powdered sample (dry weight) with 10 ml of distilled water using a roller shaker at constant rate and at room temperature for 18 h. The suspensions were then centrifuged at 3000 × g for 10 min. WAI was expressed as the weight of the wet pellet per gram of sample (g/g). WSI was expressed as the weight of dry solids in the supernatant (following evaporation to dryness at 105°C up until constant weight) and was reported as the percentage of the original sample weight.
Particle size distribution
Particle size distribution (PSD) analysis was performed on whole wheat flour samples with a low-angle laser light scattering (LALLS) using a Malvern Mastersizer S (Malvern Instruments Ltd, Worcester, UK). A sample of 0.5 g was dispersed in 10 ml of isopropanol and then sonicated for 30 s to disperse agglomerates. The sample dispersion was added to the circulating water until an obscuration of 10% to 20% was recorded. Measurement started after 1 min of agitation. Two dispersions were prepared per sample and a run was performed every minute over a 3-min period to check the stability of the dispersion. PSD were expressed as % (v/v) particles and the volume median diameter (D(v, 0.5); 50% of the distribution is above and 50% is below this value) was calculated for each population.
In vitro amylolytic digestion
In vitro starch digestibility of cereal flours was determined by monitoring the hydrolysis of each sample, after the addition of a commercial pancreatic α-amylase solution at 37°C. The colorimetric phenol–sulphuric acid method was used to determine the total amount of glucose released over time (Englyst and Cummings, Reference Englyst and Cummings1987). In particular, 60 mg (dry weight) of cereal flour were incubated in a 30 ml citrate phosphate buffer solution (0.06 mol/dm3; pH 6.9) to which was added 30 μl of commercial pancreatic α-amylase (1370 units; Sigma, Bookham, Leatherhead, UK) at 37°C. One unit of enzyme was defined as liberating 1 mg of maltose from starch in 3 min at 20°C. The level of endogenous amylase in cereal samples was also determined using the above methodology, but without the addition of exogenous amylase.
Results
In vivo responses of weaned piglets to cereal diets
Trial 1. Hard and soft wheats
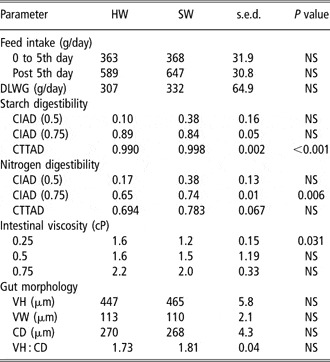
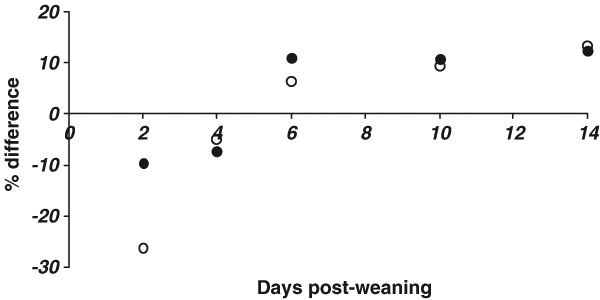
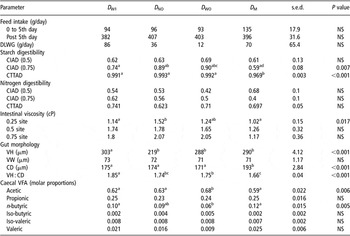
Mean results of piglet performance and intestinal measurements obtained in trial 1 are shown in Table 2. There were no significant effects of treatment on performance. Starch digestibility at the 0.5 and 0.75 sampling sites was not affected by diet, although CTTAD was significantly greater for the pigs on the soft-wheat diet (P < 0.001). There was no effect of diet on CIAD for nitrogen at the 0.5 intestinal region, but pigs on soft wheat had significantly greater coefficients at the 0.75 region (P = 0.006). CTTAD values for nitrogen were not affected by diet. Piglets fed the soft-wheat diet had intestinal digesta with a significantly (P = 0.031) less viscous supernatant fraction at the 0.25 site than pigs fed the hard-endosperm-wheat diet. Analysis of caecal digesta was not carried out in trial 1 due to a problem regarding storage of samples. Overall, no significant dietary effects were determined for any of the gut morphology parameters measured. Although villus atrophy occurred in all animals following weaning, the maximum reduction in VH observed on day 2 of the trial was smaller for the piglets fed the soft-endosperm-wheat diet (Figure 1).
Performance parameters and intestinal measurements (mean and standard error of difference (s.e.d) for 10 pigs per diet) of piglets in trial 1, where the raw cereal component was either hard (HW) or soft (SW) wheatFootnote †

NS = P > 0.05.
† Feed intake (FI) and daily live weight gain (DLWG), along with the coefficients of ileal (CIAD) and total tract (CTTAD) apparent digestibility, are shown. These were measured in different portions of the small intestine, where 0.25 represents the first quarter, 0.5 the second quarter and 0.75 the third quarter. Viscosity of the digesta supernatant was measured from material removed from the different portions of the gut. Values of villus height (VH), villus width (VW), crypt depth (CD) and the ratio between villus height and crypt depth (VH : CD) are shown.
Effect of endosperm texture of raw wheat on mean villus height measurements of piglets during the first 14 days post weaning (n = 10 piglets per diet; open circle: hard endosperm; closed circle: soft endosperm).

Trial 2. Soft wheat, barley, rye and triticale
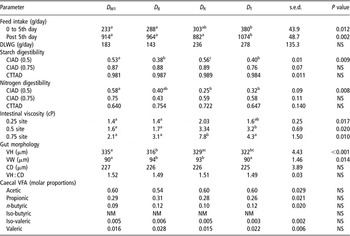
Mean piglet performance data for trial 2 are shown in Table 3. Throughout the trial period, pigs on the triticale diet consumed significantly more feed (0 to 5 days, P = 0.012; post 5 days, P = 0.002), although DLWG was not affected by dietary treatment. Starch digestibility at the 0.5 site was highest for the wheat and rye diets and lowest for the barley and triticale diets (P = 0.009). The CIAD for nitrogen at the 0.5 site was highest for the wheat diet and lowest for the rye diet (P = 0.008). No significant differences were observed for CIAD for starch or nitrogen at the 0.75 intestinal regions, and CTTAD values for starch and nitrogen were not affected by dietary cereal (P > 0.05). The rye-based diet promoted digesta with a significantly more viscous supernatant fraction at the 0.25 (P = 0.017), 0.5 (P = 0.020) and 0.75 (P = 0.010) sites. There was a significant dietary effect on VH measurements (P ⩽ 0.001) with pigs on the wheat diet having the highest mean values and animals on barley, the lowest. This situation was reversed for VW data (P = 0.014) where animals on barley and rye diets had significantly higher values than pigs on wheat and triticale diets. CD and VH : CD values were not affected by dietary treatment. Analysis of caecal digesta revealed that iso-butyric acid was absent from all samples. Molar proportions of the remaining VFAs were not affected by dietary treatment.
Performance parameters and intestinal measurements (mean and standard error of difference (s.e.d.) for 10 pigs per diet) of piglets in trial 2, where the raw cereal components were: soft wheat (D w1), barley (D B), rye (D R), or triticale (D T)Footnote †

NM = not measurable; NS = P > 0.05.
a,b,c Values within rows with different superscripts are different (P < 0.05).
† In addition to the parameters in Table 3, the levels of caecal free fatty acids (VFA) are also reported.
Trial 3. Soft wheat, maize, whole oats and naked oats
Mean piglet performance data are shown in Table 4. There was no effect of diet on mean FI but piglets in trial 3 exhibited lower average intakes than those in trials 1 and 2. DLWG values were not affected by dietary cereals, although pigs fed whole oats took an average of 7 days to regain their weaning live weight, whereas pigs on the other diets took 5 days. CIAD for nitrogen at the 0.5 and 0.75 intestinal regions and over the total tract was not affected by raw cereal type. Dietary treatment did not significantly affect CIAD for starch at the 0.5 site. However, pigs on the oat diets exhibited significantly higher CIAD values at the 0.75 region compared with animals fed the maize diet (P = 0.007). CTTAD values for starch were also significantly lower for the maize-fed pigs (P ⩽ 0.001). Viscosity of the supernatant fraction of intestinal digesta at the 0.25 site was significantly higher for piglets on the naked oat diet, compared with animals given the wheat and maize-based treatments (P = 0.017). There was no dietary difference at the 0.5 and 0.75 sections of the small intestine. Apart from VW measurements, all remaining gut morphology data were significantly affected by raw cereal type (P ⩽ 0.001). Mean VH was significantly greater for pigs fed the wheat diet, while the pigs fed a diet based on maize exhibited the highest CD and lowest VH : CD values. There was a significant effect of diet on caecal acetic acid production (P = 0.006), with the highest molar proportion from piglets fed the whole oat diet. Propionic acid levels were unaffected by dietary cereal type. Molar proportions of n-butyric acid were significantly higher (P = 0.005) in the pigs fed the maize and wheat diets, compared with animals fed a diet based on whole oats. Iso-butyric, iso-valeric and valeric acid molar proportions were unaffected by dietary treatment.
Performance parameters and intestinal measurements (mean and standard error (s.e.) for 10 pigs per diet) of piglets in trial 3, where the raw cereal components were: soft wheat (D w1), naked oats (D NO), whole oats (D WO) or maize (D M)Footnote †

In vitro characterisation of raw cereals and their corresponding diets
Trial 1. Hard and soft wheats
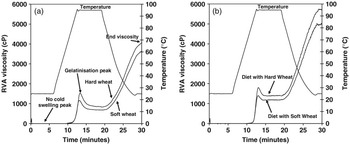
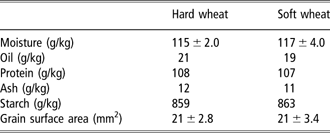
The gross composition and grain surface area of hard and soft wheats were identical (Table 5). However, the RVA pasting profiles of the two wheat flours were significantly different (P < 0.05). Higher viscosities were achieved for hard wheat compared with soft wheat on hydrating in hot water (see gelatinisation peak and end viscosity in Figure 2a). This difference was also seen for the whole diets (Figure 2b). No cold swelling viscosity was observed for the wheat samples or the whole diets. The pasting profiles of sieved wheat fractions (212 to 250 μm) also depicted higher viscosities for hard wheat than for soft wheat (results not shown). The water-holding capacity of the hard and soft wheats was very similar with low WAI (2.0 ± 0.03 and 2.0 ± 0.04 g/g, respectively) and WSI (13 ± 0.02 and 11 ± 0.28%) values exhibited. The corresponding diets showed similar WAI but elevated WSI (47 ± 2.1 and 47 ± 0.50% for hard and soft wheat, respectively) compared with those of the flours, although the WSI values were not significantly different between diets.
Rapid Visco Analyser (RVA) pasting profiles showing the temperatures and the viscosity of the pasted materials used in trial 1: (a) raw hard and soft wheat flours (10.7% dry flower in distilled water w/w) and (b) their corresponding complete diets (18.5% w/w).

Proximate analysis of raw hard and soft wheats used in trial 1

Starch was determined directly, not by difference.
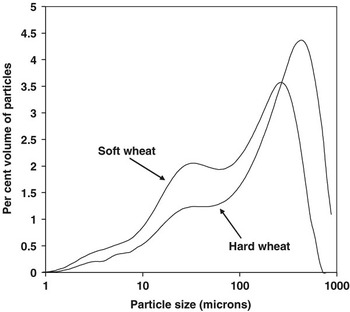
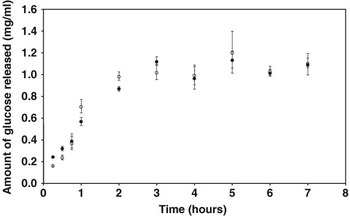
Milling and passing the hard- and soft-wheat samples through a 1.5 mm screen gave marked differences in their PSD (Figure 3). The two samples gave a bimodal distribution that consisted of a population of small particles of similar size for the two wheats (D(v,0.5) of approximately 25 μm) and a second population of particles that was bigger for hard wheat (300 ± 17 μm) than for soft wheat (212 ± 15 μm). The distribution between the two size ranges was also different, with the population of small particles (i.e. 25 μm) being predominant in the soft-wheat flour compared with the hard-wheat flour. The in vitro digestibility test was unable to differentiate between the two wheats (Figure 4).
Particle size distribution of the milled hard and soft wheats used in trial 1.

In vitro digestibility, as measured by enzymic release of glucose from the hard (closed circles) and soft (open circles) wheat flours used in trial 1.

Trials 2 and 3
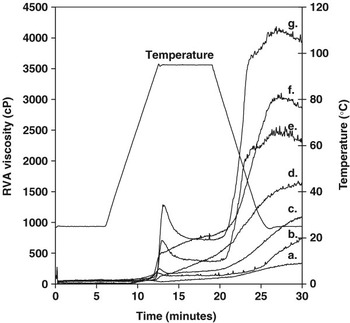
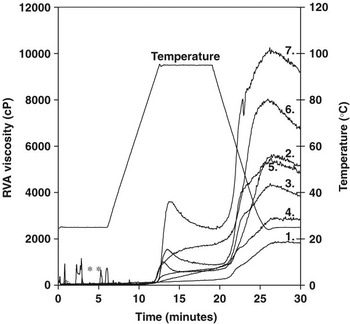
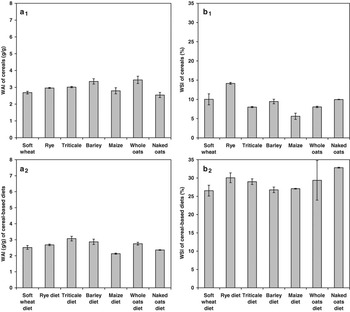
The raw cereal flours exhibited a wide range of RVA pasting profiles (Figure 5), with the end viscosities varying in the following order: naked oats > maize > whole oats > barley > triticale > soft wheat > rye. Trends for the complete diets were different from that for the cereals with the end viscosities varying in the following order: naked oats > maize > soft wheat > whole oats > triticale > barley > rye (Figure 6). No cold swelling viscosity was observed for cereals or the whole diets. All cereals and diets exhibited low and very similar WAI (approximately 3 g/g; Figure 7a1 and a2). Most cereals showed a low WSI of 8% to 10%, which is typical of raw cereals (Figure 7b1), while maize and rye had the lowest (6 ± 0.8%) and highest (14 ± 0.2%) value, respectively. In contrast, the diets displayed elevated (26% to 33%) and very similar WSI (Figure 7b2).
Rapid Visco Analyser (RVA) pasting profiles of raw cereal flours used in trials 2 and 3 (10.7% dry flour in distilled water w/w) (a. rye; b. soft wheat; c. triticale; d. barley; e. whole oats; f. maize; g. naked oats).

Rapid Visco Analyser (RVA) pasting profiles of cereal diets used in trials 2 and 3 (18.5% dry diet in distilled water w/w) (1. rye; 2. soft wheat; 3. triticale; 4. barley; 5. whole oats; 6. maize; 7. naked oats. *Indicates artefacts).

Differences in (a) the water absorption indices (WAI) and (b) the water solubility indices (WSI) between (1) cereals and (2) diets used in trials 2 and 3.

Endogenous amylase activity
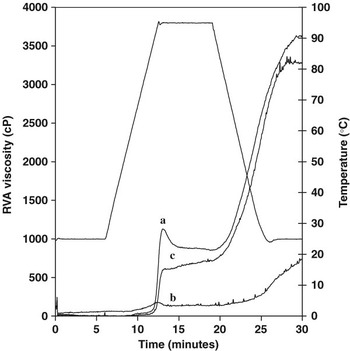
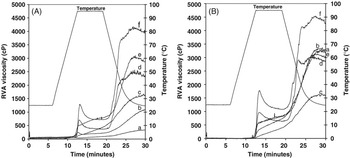
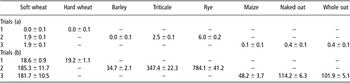
The pasting profiles of the soft wheat used in trials 2 and 3 were identical but were considerably lower than that of the soft wheat used in trial 1 (Figure 8). They however approached the profile obtained in trial 1 when the amylase inhibitor silver nitrate was added (Figure 8), although the gelatinisation peak was not fully recovered. Differences between the pasting profiles of other cereals (whole oats, naked oats, rye, triticale) before and after addition of silver ions were also identified, although not for all cereals (maize, barley) (Figure 9a and b). Endogenous amylase activities of all cereals used are shown in Table 6a and b and followed the same trend, regardless of the methodology used.
Rapid Visco Analyser (RVA) pasting profiles of (a) soft wheat used in trial 1 (in water), (b) soft wheat used in trials 2 and 3 (in water) and (c) soft wheat used in trials 2 and 3 (in AgNO3 solution).

Rapid Visco Analyser (RVA) pasting profiles of the cereal flours (a. rye; b. triticale; c. barley; d. whole oats; e. maize; f. naked oats) in the absence (A) and in the presence (B) of silver nitrate.

Endogenous amylase activity in tested cereals

(a) Expressed as the ratio [(PVAg−PVH2O)/PVH2O], where (PVAg) is the RVA pasting parameter of peak viscosity determined in AgNO3, and (PVH2O) is that determined in water).
(b) Expressed in μg of released glucose/g of sample per ml.
Discussion
The current work applies a new experimental approach consisting of fully characterising the physicochemical properties of cereals and diets, and relating these measurements to the biological responses of weaned piglets upon feeding.
Trial 1. Hard and soft wheats
Previous work examining the effect of wheat cultivar on pig performance has failed to show a clear relationship with digestibility (Pearce et al., 1997; Lewis et al., 1999). It is important to note that the current trial quantified endosperm hardness, in contrast to previously published reports that rely only on an official ‘hardness’ description supplied by breeders/UK National Institute of Agricultural Botany as an aid to growers. For the initial 5 days of the trial, no dietary influence on FI could be established. This is not surprising since voluntary FI of piglets in the period immediately following weaning is often highly variable (Bark et al., Reference Bark, Crenshaw and Leibbrandt1986). However, following the initial 5-day period, there was a tendency (P = 0.063) for piglets fed soft wheat to consume more feed.
Analysis of biological responses between weaned piglets in trial 1 revealed no dietary effect on a number of other parameters such as daily live weight gain (DLWG) or mean gut morphology. The absence of an effect of endosperm texture on DLWG supported the findings of Pearce et al. (1997). This may initially suggest that endosperm texture alone is not paramount in determining the nutritional value of wheat when all other cereal characteristics (e.g. protein, fat and starch levels, environmental factor) are identical between cereals. However, endosperm texture contributes considerably to the milling behaviour of wheat (Haddad et al., Reference Haddad, Mabille, Mermet, Abecassis and Benet1999), and hence to the hydration properties of wheat flour. The amount of starch damage inflicted by the milling procedure is generally low. The fracture planes in soft grains tend to traverse endosperm cells and follow the interface between the starch granule surface and the surrounding protein matrix, suggesting that mechanical damage to the granules due to milling should be minimal.
By contrast, the fracture planes in hard grains are located along the lines of the cell boundaries, requiring higher shearing forces for milling, which can cause more mechanical damage to the granules. This suggests that milling can cause characteristic differences between hard and soft wheats, such as PSD, particle shape and damage to starch granules. The present study showed that soft-wheat flour had smaller particles sizes compared with hard-wheat flour, which is in agreement with previously published work (Glenn and Saunders, Reference Glenn and Saunders1990; Devaux et al., Reference Devaux, Le Deschault de Monredon, Guibert, Novales and Abecassis1998). This finding can partly explain the differences in hydration and viscous properties of the samples shown by the RVA. In particular, the hard-wheat flour, with some starch damage and large particles, had a higher viscosity when placed in hot water. The amount of milling of the raw starches could alter the behaviour of the product when digested, for example the damaged starch would readily hydrate and be digested, but the majority of the material would be encased in particles that would be difficult to hydrate, thereby lowering the rate of digestion. This suggests that hard wheat may be less favourable for the weaned piglet than soft wheat. This is partly supported in the piglet data from trial 1 where feeding a soft-wheat diet resulted in a less viscous supernatant digesta fraction (at the 0.25 region) and increased apparent digestibility of starch and nitrogen.
It should be noted that, although no dietary differences in viscosity were determined at the remaining intestinal regions, the supernatant viscosity analysis method does not account for the properties of particulate material and its contribution to complete, intact digesta viscosities. It is therefore most probably not suitable to differentiate between the two wheat cereals. The usefulness of this method has already been questioned elsewhere (Takahashi and Sakata, Reference Takahashi and Sakata2002 and Reference Takahashi and Sakata2004) and a recommendation is made to apply recently developed and validated methodologies analysing whole digesta viscosity in future studies (E. Lee, F.J. Doucet, S.E. Hill and J. Wiseman, unpublished findings).
Regardless of endosperm texture, feeding a diet based on unprocessed wheat caused a collapse in starch digestibility immediately post weaning in both the mid (0.5) and distal (0.75) regions of the small intestine, particularly pronounced in the former. This observed reduction in starch digestion in the days immediately following weaning could contribute to the commonly observed post-weaning growth check in weaned piglets (Doucet et al., Reference Doucet, White, Wiseman and Hill2007) that is typically associated with a deterioration in health status.
This drop in starch digestion coincided with the observation of a typical pattern of villus atrophy immediately following weaning. All animals experienced maximum reduction in VH (when compared against values of the control piglets on day 0 of weaning) around day 2 to 4 post weaning, before progressively recovering to pre-weaning levels by day 5. Villus atrophy was however found to be less severe for piglets fed soft wheat. There is considerable evidence in the literature to suggest that the physical presence of food within the gastrointestinal tract plays a strong role in the integrity of the structure and function of the small intestine after weaning (Kelly et al., Reference Kelly, Smyth and McCracken1991; Pluske et al., Reference Pluske, Williams and Aherne1996; Spreeuwenberg et al., Reference Spreeuwenberg, Verdonk, Gaskins and Verstegen2001). In trial 1, however, FIs between wheats were not significantly different during the experimental period. Therefore, gut morphology results from the current trial appear to suggest an interaction between villus architecture and wheat endosperm texture in the immediate post-weaning period. A degree of caution should be made, however, when assessing the significance of this observation, due to the limited number of piglets analysed per diet on each slaughter day. A recommendation to select soft-wheat cultivars for piglet feeding would emerge from the data presented, although further comparative studies are needed. Future work should include a wider range of wheat cultivars with varying endosperm texture, and a larger sample population on each slaughter day. Such comparative studies would also benefit from using in vivo animal responses and in vitro rheological tests together.
Trial 2. Soft wheat, barley, rye and triticale, and Trial 3. Soft wheat, maize, whole oats and naked oats
The high variability of in vivo starch digestibility between cereals most likely depends on the source and nature of starch (Aarathi et al., Reference Aarathi, Urooj and Puttaraj2003). However, the primary properties affecting starch digestibility amongst cereals remain unclear owing to the complexity of the starch structure and variation in composition within a specific cereal type (Svihus et al., Reference Svihus, Uhlen and Harstad2005). The content of endogenous amylase in cereals has been substantially overlooked as a variable, as illustrated by the limited number of animal studies that have measured this parameter.
The present study provides, for the first time, two strong indications that the content of endogenous amylase in cereals may be of greater importance than originally thought, although this conclusion is based substantially on comparisons between the two soft-wheat samples evaluated. First, the presence of endogenous amylase in the soft wheat used in trials 2 and 3, but not in the soft wheat used in trial 1 (Table 6a and b), strongly affected the hydration characteristics of the cereal, as shown by the RVA pasting profiles. This is despite having used the same variety of soft wheat, grown by the same breeder at the same site, but harvested on 2 consecutive years. Consequently, although the soft wheat was originally used in all three trials as a control, the observed variation in endogenous amylase content and the resulting significant differences in the physicochemical properties of the wheat starches between trials was an important feature of the current study. Second, endogenous amylase was identified in varying, and often non-negligible, amounts in some, but not all cereals used in trials 2 and 3 (Table 6a and b). This resulted in the undesired introduction of an additional variable in the study, which made direct comparison between the physicochemical properties of cereals and between their nutritional values in piglets difficult.
Although digesta supernatant viscosity was affected by dietary cereal in trial 2, the range of values measured was fairly low and did not have a negative effect on piglet performance in the first 2 weeks post weaning. A typical pattern of villus atrophy and recovery was seen for all pigs in the period following weaning. Although significant dietary effects were identified for VH and VW measurements, there was no clear correlation with cereal type. An interesting observation from the soft wheat used in trial 2 (compared with the batch of soft wheat used in trial 1) was that the elevated endogenous amylase activity measured in vitro was found to correlate positively with a higher apparent digestibility of starch at the 0.5 intestinal region. These findings suggest that the presence of endogenous amylase in wheats may accelerate the rate of starch digestion in the small intestine, although further investigations are required to elucidate the potential benefit(s)/disadvantage(s) of elevated amounts of endogenous amylase in wheats used in animal feeds.
A similar correlation to that found in trial 2 was also identified in trial 3. Once again, the elevated endogenous amylase activity of the soft wheat used (identical wheat batch to that used in trial 2) appeared to correlate with a higher apparent starch digestibility at the 0.5 region of the small intestine. It could be expected that the presence of endogenous enzyme would have no bearing on the digestibility pattern of native starches. Endogenous piglet amylases could be expected to be plentiful and would readily break down susceptible starches. However, there is some indication that starches that have already undergone some enzymic degradation are more rapidly digested. This finding supports the above line of reasoning whereby endogenous amylase in wheat may well encourage in vivo starch digestibility in the small intestine of weaned piglets and, as such, would warrant further research.
In agreement with the observations made in trials 1 and 2, apparent starch digestion within the small intestine increased from the mid to distal region for three of the four cereals examined in trial 3. Analysis of gut morphology data revealed that piglets fed the soft-wheat diet had significantly higher VH values (P ⩽ 0.001), suggesting that the soft wheat might therefore be considered to be beneficial, compared with the other cereals examined. There is no immediate explanation for the differences found in VH between the soft wheats in the three trials. Although not statistically significant, the whole-oat diet resulted in the lowest levels of propionic acid in the caecum. This can be explained by the same treatment group having the highest CIAD values for starch within the 0.5 and 0.75 sites of the small intestine, indicating that less starch was available for fermentation for propionic acid within the hind gut. In addition, the low DLWG values observed and the increased number of days taken post weaning to achieve pre-weaning live weight values suggest that whole oats was the least favourable dietary cereal for the young piglet.
Conclusion
The variation in piglet data and in the control diets makes it more difficult to come to a conclusion about the suitability of the different cereals as major ingredients in diets for newly weaned pigs. Atrophy of the villi was seen in all animals in the days immediately following weaning – an observation typically associated with weaning anorexia at this time. However, the fact that piglets on the soft wheat showed the highest comparative villi heights in each of the three trials, yet there was no correlation with FI data, suggests there may also be an interaction between raw cereal type and villus architecture in the immediate post-weaning period.
Soft wheats were run as a control diet in all three trials. Care was taken to ensure the same variety was used from the same grower. If in vitro testing had not been performed, the variation in endogenous amylase content would not have been identified. The fact that differences were found in endogenous amylase activity between wheat batches, and that this could be correlated with the 0.5 starch digestibility data, suggests that endogenous amylase content could be an important variable within wheats. As such, future nutritional studies on wheat may benefit from a pre-characterisation step of the selected wheats in terms of endogenous amylase activity. The results also highlight the necessity of performing in vitro assessment of diets to characterise fully the properties of starch sources prior to undertaking animal trials.
Acknowledgements
This research was financially supported by ABNA Ltd, Frank Wright Ltd, Home-Grown Cereals Authority, Meat and Livestock Commission/British Pig Executive, Primary Diets Ltd and Provimi Ltd, with match funding from Defra, through the Sustainable Livestock Production LINK programme.