


Introduction
An imbibed seed that is dried before germination is complete will not survive if imbibition has proceeded beyond a critical fraction of the total time required for germination (Evenari et al., Reference Evenari, Shanan and Tadmor1971; Hong and Ellis, Reference Hong and Ellis1992; Lin et al., Reference Lin, Yen and Chien1998; Reisdorph and Koster, Reference Reisdorph and Koster1999). Once a seed has gone beyond this critical ‘point of no return’ (Evenari et al., Reference Evenari, Shanan and Tadmor1971), it is committed to germination and subject to the risks of a subsequent change in environmental conditions. Thus, the germination process is an unusual event in the life cycle of a plant because it represents a binomial as opposed to a graduated response to the environment.
For orthodox, desiccation-tolerant seeds, the loss of desiccation tolerance during germination increases the risk of this already high-risk stage in the plant's life cycle. The risk associated with desiccation during germination can be spread by producing large numbers of seeds, by shedding these over an extended period (Garwood, Reference Garwood1983) and by producing a population of seeds that have a range of times to germination (Harper, Reference Harper1977). These strategies allow plants to increase the probability that some seeds will complete germination and emerge in conditions that favour establishment. There is a considerable body of literature on the first two of these strategies, but less attention has been paid to the significance of the distribution of times to germination, or of the critical imbibition proportion (i.e. when desiccation tolerance is lost during germination) and implications this may have for seed survival in field conditions. In addition, we do not know if the critical fraction of the germination time, beyond which desiccated seeds do not survive (hereafter referred to as the critical imbibition proportion, CIP), varies within a seed population and whether it varies between species.
The survival of previously imbibed seeds after desiccation might be particularly important in seasonally dry environments, where the onset of the wet season is preceded by rainfall events of irregular timing and amount. For example, at our study site in tropical semi-evergreen rainforest on Barro Colorado Island (BCI), Panamá, seed dispersal of pioneer trees takes place predominantly during the 4-month dry season (see Table 1), but germination and seedling emergence are concentrated at the beginning of the wet season (Garwood, Reference Garwood1983; Daws et al., Reference Daws, Pearson, Burslem, Mullins and Dalling2005). However, the transition from dry to wet season consists of an increasing frequency of high rainfall events, rather than an abrupt change from a low to high rainfall regime (Daws, Reference Daws2002). Furthermore, following a few days of soil drying in large canopy gaps, soil matric potential (SMP) close to the soil surface can fall from field capacity ( − 5 kPa) to below the permanent wilting point ( − 1.5 MPa) (Engelbrecht et al., Reference Engelbrecht, Dalling, Pearson, Wolf, Gálvez, Koehler, Tyree and Kursar2006; Daws et al., Reference Daws, Ballard, Mullins, Garwood, Murray, Pearson and Burslem2007). In these circumstances, seeds of pioneer trees in canopy gaps and close to the soil surface are likely to be exposed to cycles of imbibition and desiccation prior to the onset of the wet season. Thus, for species that germinate rapidly, there is a potential risk of high mortality of imbibed seeds if desiccation occurs subsequently, although differences among species with respect to the risk of seed mortality have not been investigated. This risk is in addition to the risk of desiccation of recently germinated seedlings, whose radicle is overtaken by the soil drying front (Daws et al., Reference Daws, Ballard, Mullins, Garwood, Murray, Pearson and Burslem2007). Differences in CIP among species provide a mechanism for differential establishment success in response to variation in SMP. In forest ecosystems, variation in SMP is associated with gradients of gap size and canopy openness (Becker et al., Reference Becker, Rabenold, Idol and Smith1988; Veenendaal et al., Reference Veenendaal, Swaine, Agyeman, Blay, Abebrese and Mullins1995), topography (Becker et al., Reference Becker, Rabenold, Idol and Smith1988; Daws et al., Reference Daws, Mullins, Burslem, Paton and Dalling2002b) and inter-annual differences in rainfall. Thus, spatio-temporal variation in SMP may contribute to the maintenance of species richness if coexisting species differ substantially in their germination characteristics. Consequently, the aims of this work were to determine the timing of the loss of desiccation tolerance during germination and to test whether the CIP varies within and between species. Since the timing of the loss of desiccation tolerance has implications for the proportion of seeds in a population that can be killed by drying, we also explore the relationship between: (1) the CIP and the maximum proportion of seeds in a population that can be killed by a single drying event, and (2) the effect of the population-level germination characteristics (slope of the germination curve and time to 50% germination) on the maximum proportion of seeds in a population that can be killed by a single drying event. These questions were addressed by studying the response to desiccation of selected tropical pioneer species (sensu Swaine and Whitmore, Reference Swaine and Whitmore1988) that differ in their distribution across forest gap environments.
Some characteristics of the study species and fitting constants for the Hill function G(t)=at b/(t 50b+t b), which was fitted to the control (non-desiccated) germination progress curves. Family names lack the –aceae suffix

# From Croat (Reference Croat1978); ***P < 0.001; †maximum germination fraction.
Theory
Let the proportion of a population of seeds that germinate under a non-limiting water supply after a time t, be G(t). If these seeds have been imbibed for a time t and then desiccated, G(t) of the seeds have already germinated, but the remaining seeds are split between: (1) a fraction M(t) so close to germination that they are killed by desiccation; and (2) those seeds that can still germinate on rewetting. Let Δ be the additional time that would have been required to germinate the killed seeds if they had not been desiccated (see Fig. 1). Then the proportion M(t), of the ungerminated, desiccated seeds (relative to the total germinable seeds in the seedlot) that fail to germinate after rewetting is:
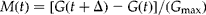
where G max is the maximum proportion of seeds that germinate under normal conditions.
Schematic summarizing the response of a hypothetical population of seeds, with maximum germination of G max (a in Hill function), to a drying event at time t during imbibition. Thus, seeds in the population can be divided into three categories: (1) those that germinate pre-desiccation, G(t)/G max; (2) those that are sufficiently close to germination that are killed by desiccation, M(t); and (3) those that can still germinate after re-imbibition, P(t).

Assume that the proportion of seeds represented by M have been wetted for a fraction ≥ y of their full germination time, where y, the critical imbibition proportion (CIP), is a constant and is the same for all seeds in the population. Then

Substituting this into equation (1) gives
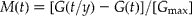
and the proportion, P(t) of the population that remain germinable after desiccation, 1 − M(t) − [G(t)/G max] is
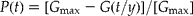
Thus, if the functions G(t) and P(t) have been experimentally determined, it is possible to determine y by a process of optimization in which y is allowed to vary until the best fit between the experimental P(t) and that predicted by equation (4) is obtained.
Materials and methods
Study site and seed lot details
Seeds of eight pioneer tree species (see Table 1) were collected from semi-deciduous forest on Barro Colorado Island (BCI), Republic of Panamá (9°10′N, 79°51′W) between February and April 1999. Seeds of the ninth study species, Cecropia longipes, were collected in July 1999. The flora and vegetation of BCI are described in detail elsewhere (Leigh et al., Reference Leigh, Rand and Windsor1982; Leigh, Reference Leigh1999). Annual rainfall on BCI averages 2600 mm yr− 1, with a pronounced dry season between January and April (Dietrich et al., Reference Dietrich, Windsor, Dunne, Leigh, Rand and Windsor1982). For all species, intact fruits were collected from at least five separate trees. Seeds were separated from fruit tissue and air-dried in the dark, prior to being air-freighted to Aberdeen, UK in polystyrene containers. In the UK, seeds were stored at room temperature in the dark prior to the commencement of germination experiments.
Seed desiccation tolerance following imbibition
Seeds of the study species were sown in 50 mm Petri dishes (3 × 40 seeds per species) on two layers of Whatman No. 42 filter papers, wetted with distilled water. Petri dishes were placed in a growth chamber (Fi-totron 600H, Fison Environmental Equipment, Loughborough, UK) at 26 °C and a ratio of red:far-red light (R:FR) of 2 (12 h day/12 h night). Prior to sowing, Apeiba tibourbou and Ochroma pyramidale seeds were soaked in hot water at 80 or 90°C, respectively, for 2 min, to enable subsequent water uptake (Acuna and Garwood, Reference Acuna and Garwood1987; Daws et al., Reference Daws, Orr, Burslem and Mullins2006).
For the control (non-desiccated) treatment, germination was scored every 24 h, with germination defined as visible radicle emergence. Based on the time to germination for each species, additional dishes of seeds were allowed to imbibe for a range of intervals up to the completion of germination. At each of these pre-determined time points, three Petri dishes of seeds per species were randomly selected, and the filter papers and seeds were removed from the Petri dishes and left in the growth chamber to desiccate for 4 d to simulate the occurrence of soil drying. Relative humidity in the growth chamber was c. 40% and was measured with a sensor (SKH 2065, Skye Instruments, Llandrindod Wells, UK) attached to a datalogger (Datahog, Skye Instruments). Seeds of all species reached constant mass within 2 h of the start of drying. After drying, the filter papers (and seeds) were placed back in Petri dishes, re-wetted with distilled water and monitored for germination daily.
Statistical analyses
A Hill function was fitted to the germination progress curves for the nine species using Sigma Plot 7 (SPSS Inc., Chicago, Illinois, USA). Thus:

where G(t) is germination as a function of time (t) and a, b and t 50 are fitting constants. The Hill function has several advantages for describing germination progress curves. In particular, a corresponds to the maximum observed level of germination and t 50 is the time to 0.5 of maximum germination; b is the slope parameter. However, b does not correspond to the actual slope of the germination curve. For the purposes of understanding how the actual slope (d− 1) of the curve impacts on seed mortality, the Hill function was differentiated such that

describes how the slope of the germination curve changes with respect to time (t).
Using the species-specific parameters for each of the nine study species (Table 1), equation (5) was used to predict values of G(t) and G(t/y) for a range of values of y (critical imbibition proportion; CIP) between 0.0 and 1.0. These predicted values were then substituted into equation (4) to predict P(t). Estimated values of P(t) from equation (4), corresponding to the times when desiccation occurred, were then plotted against experimentally determined values of P(t), varying y until the best fit (smallest residual variance) using least squares linear regression (implemented in Minitab 13; Minitab Inc., Pennsylvania, USA) was obtained. The value of y that gave the best fit was taken as the proportion of the germination time after which seeds lose their desiccation tolerance (CIP).
Subsequently, we investigated how changes in CIP, t 50 and maximum slope of germination progress curves affect the maximum proportion of seeds that can potentially be killed by a single drying event during imbibition (M max), i.e. the worst-case scenario for seed mortality from a single drying event. All three of these parameters are potentially subject to selection. Consequently, we aimed to define the ‘optimum’ set of characteristics that would minimize potential mortality. First, to determine how changes in CIP affect mortality, we used equation (5) with parameters that corresponded to a germination proportion of 1, a t 50 = 10 d and maximum slope of 0.1 d− 1. The value of b [slope parameter in equation (5)] corresponding to a maximum slope of 0.1 d− 1 was calculated using equation (6) to determine the maximum slope of the germination curve as b was varied. These values were chosen because they are within the observed range of these parameters for the nine study species (Table 1). G(t/y) was then calculated using equation (5) for values of y from 0 to 1 in 0.05 increments. This was substituted into equation (3) for values of t from 0 to 30 d, to determine how the proportion of seeds [relative to the total seedlot; equation (3)] that could potentially be killed by desiccation changed with t. This enabled M max to be identified. Similarly, for a value of y of 0.66 (the mean value across the nine study species), values of b and t 50 in the Hill function [equation (5)] were changed to determine the effect of varying t 50 and slope on M max. Again, the value of b to use for each slope was determined by using equation (6) to determine the relationship between b and slope (d− 1).
Results
Timing of the loss of desiccation tolerance
Cumulative germination of the study species was sigmoidal, with a Hill function providing a highly significant fit to the relationship between cumulative germination and time for each species (R 2>0.99, P < 0.001; Fig. 1, Table 1). In addition, as germination of each species progressed, the number of seeds killed by desiccation first increased and then decreased. The maximum proportion of seeds susceptible to desiccation occurred shortly before germination of the population reached 0.5 (Fig. 2).
Germination progress curve for Cecropia longipes (closed circles) and the proportion of seeds killed by desiccation following various periods of imbibition (open circles).

For the nine species, determination of the CIP by iteration resulted in a value between 0.6 and 0.7 (Table 2); this value corresponded to the CIP that maximized the R 2 of the relationship between the predicted numbers of seeds to germinate post desiccation versus actual germination post desiccation (Fig. 3). In addition, for all nine species the linear relationship between actual and predicted survival post desiccation was highly significant (R 2 > 0.94, P < 0.001), indicating that the CIP was relatively constant for all seeds within each population.

Predicted [from equations (4) and (5)] versus actual germination of seeds of Cecropia longipes for the best value (value that gives the best match between actual and predicted values of germination) of y (critical imbibition proportion, CIP) of 0.66 (filled circles). For comparison the actual versus predicted germination for a CIP of 0.2 (open squares) and 0.9 (open triangles) are presented. These data demonstrate the lack of a fit of the predicted to actual data when using values of CIP that differ from the optimized value (0.66). The dashed line is a 1:1 null line, and the solid line is a fitted linear regression to the data for a CIP of 0.66.

Effect of germination parameters on potential seed mortality
Equation (3) was used to calculate the maximum proportion of imbibed seeds that could be killed by desiccation, in hypothetical populations of seeds differing in CIP. For a population of seeds with a germination fraction of 1.0, a t 50 of 10 d and maximum slope of the progress curve of 0.1 d− 1, the maximum proportion of the population that could be killed by desiccation (i.e. drying at the most susceptible time point during imbibition) was close to 1 for a CIP of between 0 and 0.1 and then steadily decreased to 0 as CIP increased to 1 (Fig. 4).
The effect of varying the critical imbibition period on the fraction of seeds in a population that can be killed by a single desiccation event during imbibition (M max). Parameters used in the Hill function [equation (5)] were 1.0, 3.6 and 10 for a, b and t 50, respectively, corresponding to a maximum germination fraction of 1.0 and a maximum slope of 0.1 d− 1.

For a constant CIP of 0.66 (the mean value across the study species), M max increased with increasing t 50 and maximum slope of the germination progress curve (Fig. 5). For example, for a slope of 0.2 d− 1, M max increased from c. 0.1 to 0.9 as t 50 increased from 3 to 25 d (Fig. 5). Similarly, for a t 50 of 20 d, as the slope increased from 0.03 to 0.25 d− 1, M max increased from c. 0.13 to 0.95 (Fig. 5). Superimposing the nine study species on Fig. 5 revealed that although the species varied in t 50 and slope, M max was in the region of 0.45–0.60 (i.e. as t 50 increased for the study species, the slope of the germination curve decreased).
The effect of germination progress curve shape (as defined by t 50 and maximum slope) on the maximum proportion of seeds that can be killed in a population by drying during imbibition (M max), assuming a critical imbibition period of 0.66 (the average value across the nine study species). Numbers adjacent to the lines refer to the maximum slope of the germination progress curve (d− 1). Downward triangles correspond to data for the nine study species.

Discussion
For nine species from semi-deciduous tropical forest in Panamá, seeds were killed by drying during imbibition. For each species, all individual seeds in the population became sensitive to drying after germination had progressed to a fixed proportion of their germination time. This proportion of a seed's germination time after which desiccation tolerance is lost, was also relatively constant across species (CIP of 0.6–0.7). Thus, the proportion of seeds in a seedlot that are at greater than c. 0.66 of their germination time (and have not already germinated) defines the fraction of the seedlot that could potentially be killed by a single drying event. Across the nine species, the maximum proportion of the seedlot that could be killed by such an event (M max) was 0.47–0.64. Figure 5 demonstrates that the proportion of seeds in a population at >0.66 of their germination time that can be killed by desiccation increases with t 50 and with the slope of the germination curve. However, since slope decreases as t 50 increases (Fig. 5) for the nine species, the two effects tend to offset one another.
Implications for seed mortality
Orthodox, desiccation tolerant seeds lose desiccation tolerance during germination (Hong and Ellis, Reference Hong and Ellis1992), and this occurs close to the onset of visible germination (Hong and Ellis, Reference Hong and Ellis1992; Lin et al., Reference Lin, Yen and Chien1998; Buitink et al., Reference Buitink, Leger, Guisle, Vu, Wuilleme, Lamirault, Le Bars, Le Meur, Becker, Küster and Leprince2006). The present work not only quantifies the timing of this loss of desiccation tolerance, but also shows that all seeds in a seed population have similar responses when the duration of imbibition is considered on a proportional basis. Furthermore, while previous studies have correlated the loss of desiccation tolerance with particular biochemical and physiological events during germination (Osborne and Boubriak, Reference Osborne and Boubriak1994; Boubriak et al., Reference Boubriak, Kargiolaki, Lyne and Osborne1997; Lin et al., Reference Lin, Yen and Chien1998; Buitink et al., Reference Buitink, Leger, Guisle, Vu, Wuilleme, Lamirault, Le Bars, Le Meur, Becker, Küster and Leprince2006), the implications for seed mortality in the field have been overlooked. Conversely, studies on seed and seedling survival in the field have typically focused on mortality resulting from pathogenic fungi (Augspurger, Reference Augspurger1983; Dalling et al., Reference Dalling, Swaine and Garwood1998) and the death of newly emerged seedlings caused by drought (Augspurger, Reference Augspurger1979; Blain and Kellman, Reference Blain and Kellman1991; Engelbrecht et al., Reference Engelbrecht, Dalling, Pearson, Wolf, Gálvez, Koehler, Tyree and Kursar2006). In contrast, our data suggest that desiccation during germination may represent a significant agent of mortality for seeds in the soil seed-bank.
Desiccation tolerance can be re-induced in germinating seeds of a few species (e.g. cucumber, Impatiens and Medicago truncatula; Bruggink and van der Toorn, Reference Bruggink and van der Toorn1995; Buitink et al., Reference Buitink, Vu, Satour and Leprince2003). Although this process could reduce the impact of seed mortality from desiccation, the re-induction of desiccation tolerance requires highly specific conditions (i.e. constant water potentials of c. − 1.5 MPa; Bruggink and van der Toorn, Reference Bruggink and van der Toorn1995; Buitink et al., Reference Buitink, Vu, Satour and Leprince2003) and occurs during a very narrow developmental window (Buitink et al., Reference Buitink, Leger, Guisle, Vu, Wuilleme, Lamirault, Le Bars, Le Meur, Becker, Küster and Leprince2006). Therefore, it is not clear whether this process occurs under field conditions, or whether it has adaptive significance.
The rate of seed drying can affect the level of desiccation tolerance for both developing orthodox seeds and for recalcitrant, desiccation-sensitive seeds (Kermode and Finch-Savage, Reference Kermode, Finch-Savage, Black and Pritchard2002; Pammenter et al., Reference Pammenter, Berjak, Wesley-Smith, Vander Willigen, Black and Pritchard2002). However, despite nearly four orders of magnitude difference in seed mass across the present study species, and consequently likely differences in drying rates, there was no correlation between the CIP and log10(seed mass) (R 2 = 0.1, df = 7, P > 0.05), suggesting that drying rates did not affect our results.
Implications for selection on germination parameters
In these experiments, seeds have been allowed to imbibe and germinate under a daily light regime. However, when imbibed seeds of Piper auritum H.B.K. and Cecropia obtusifolia Bertol were stored in the dark at 25 °C and then exposed to light, there was no decrease in percentage germination after storage of up to 1 year (Vázquez-Yanes and Smith, Reference Vázquez-Yanes and Smith1982). Thus, it is likely that seeds of tropical pioneers can survive in a dry or imbibed state for long periods in the soil, unless attacked by predators and pathogens, and they are also able to tolerate desiccation after imbibition in the light, provided that they have only progressed partly towards germination. However, once they have exceeded a critical period of imbibition, they cannot survive desiccation. Thus, seeds of such species may be able to survive in a quiescent state for long periods when the red:far-red light ratio or soil temperature fluctuations are too low to trigger germination, because they are beneath leaf litter or are not in a sufficiently large gap (Daws et al., Reference Daws, Burslem, Crabtree, Kirkman, Mullins and Dalling2002a; Pearson et al., Reference Pearson, Burslem, Mullins and Dalling2002). They can thus await the decay or removal of litter, or the creation of a gap of sufficient size to trigger germination (Daws et al., Reference Daws, Burslem, Crabtree, Kirkman, Mullins and Dalling2002a; Pearson et al., Reference Pearson, Burslem, Mullins and Dalling2002). However, once the appropriate germination trigger is received, they are as vulnerable to desiccation and death as seeds that lack such cues. Furthermore, there is a high risk of seed desiccation during short rain-free periods that dry the top few millimetres of the soil, particularly for small-seeded pioneers that can only emerge from shallow depths (typically a few millimetres) (Bond et al., Reference Bond, Honig and Maze1999; Pearson et al., Reference Pearson, Burslem, Mullins and Dalling2002). Therefore, it is important that their distribution of germination times is optimized to minimize the probability of mortality.
Thus, the loss of desiccation tolerance after 0.6–0.7 of the time to visible radicle emergence might be expected to result in selection to modify germination parameters (CIP and the shape of the germination curve; t 50 and slope) to minimize, at any given time during imbibition, the proportion of seeds that have progressed beyond the CIP and can be killed by drying. Figure 4 suggests there will be selection for the CIP to be close to 1 (i.e. late in the germination process), which would minimize the proportion of the seed population that would be vulnerable to drying. However, a value of c. 0.66 may be an unavoidable constraint imposed by the germinating embryo, as it functionally becomes a seedling (and hence desiccation sensitive), prior to visible germination (radicle emergence). It would clearly be useful to discover whether such a narrow range of CIPs is applicable to a wider range of species, including species from arid environments.
In addition, for a given slope, a larger proportion of seeds of slow (high t 50) germinating species will be killed than seeds of rapidly (low t 50) germinating species (Fig. 5). Consequently, this predicts that the maximum slope of germination curves should also decrease with increasing t 50, which would minimize the proportion of seeds that can be killed (Fig. 5). This prediction is supported by data for the nine study species (Fig. 5); there was a significant negative correlation between t 50 and slope (R 2 = 0.759, df = 7, P < 0.001). Thus, seed mortality resulting from desiccation provides a potential explanation for the observed trend of an increasing spread of germination times with increasing t 50. However, this pattern might also reflect inevitable consequences of the kinetics of germination; further studies are required to examine the selection pressures operating on germination kinetics across diverse taxa to test whether this is either a general relationship or restricted to species from water-stressed environments.
This also raises the question of why species differ in their time to germination (t 50). In addition to seed mortality, one explanation is that a trade-off between seedling mortality and germination micro-site pre-emption provides a selective pressure on germination times. Thus, in areas with unpredictable rainfall, there may be selection for slow (and spread out) germination times to reduce the risk of high seedling mortality (Thanos et al., Reference Thanos and Doussi1995a, Reference Thanos, Kadis and Skaroub; Doussi and Thanos, Reference Doussi and Thanos2002) (i.e. seedling emergence does not occur rapidly after small, isolated rainfall events when rapid soil drying could result in high seedling mortality). In contrast, rapid germination following rainfall has the advantage of maximizing the length of the growing season and allowing site pre-emption in advance of slower germinating species (Garwood, Reference Garwood1983; Daws et al., Reference Daws, Pearson, Burslem, Mullins and Dalling2005). Such behaviour has been selected for in many cultivated crops (Smith, Reference Smith1998), and is also likely to operate for these pioneer species. The fastest germinating species (lowest t 50; Table 1) occur preferentially in large canopy gaps (Croat, Reference Croat1978; Dalling et al., Reference Dalling, Lovelock and Hubbell1999; Pearson et al., Reference Pearson, Burslem, Goeriz and Dalling2003) where soil drying is most rapid (Veenendaal et al., Reference Veenendaal, Swaine, Agyeman, Blay, Abebrese and Mullins1995), and are the largest seeded (O. pyramidale, L. seemannii, A. membranacea and A. tibourbou). For these species, the risk of seedling mortality from soil drying is reduced by a fast radicle growth rate (Daws et al., Reference Daws, Ballard, Mullins, Garwood, Murray, Pearson and Burslem2007) and an ability to emerge from greater soil depths than smaller-seeded species (Pearson et al., Reference Pearson, Burslem, Mullins and Dalling2002). Consequently, an advantage of fast germination is rapid growth and micro-site pre-emption in the high light environment of large gaps. In contrast, potentially high seedling mortality of small-seeded species may select for slower germination, which is coupled with a shallow slope of the germination progress curve. Indeed, for the nine study species, there was a significant negative relationship between t 50 and log10(seed mass) (R 2 = 0.54, df = 7, P = 0.025).
In conclusion, for nine neo-tropical pioneer species, seed desiccation tolerance is lost at a constant proportion of individual seed time to germination, with this value being fairly constant across the species. Thus, for these pioneer species, this study suggests that the risk period from drought for seedlings not only applies post germination as has been shown previously (e.g. Engelbrecht et al., Reference Engelbrecht, Dalling, Pearson, Wolf, Gálvez, Koehler, Tyree and Kursar2006), but also extends to before visible germination, if germination has progressed beyond the CIP. Further work to determine the implication of the loss of desiccation tolerance on seed mortality in the field for seeds of a wider range of t 50, and those germinating under various rainfall scenarios, is required.
Acknowledgements
We thank the Natural Environment Research Council for funding (studentship to M.I.D.). The Royal Botanic Gardens, Kew is supported grant-in-aid from Defra. Drs J.W. Dalling, J.B. Dickie, I. Kranner and H.W. Pritchard provided helpful comments that significantly improved the manuscript.



