1. Introduction
Flapping-wing micro air vehicles (FWMAVs), compared to fixed-wing/rotor, possess superior miniaturized aerodynamic theory, lower noise, and stronger resistance to turbulence [Reference Abas, Rafie and Yusoff1, Reference Xu, Pan and Xu2]. It plays a key role in military and civilian fields [Reference Kim, Hong and Im3]. However, the lack of takeoff capability and difficulty in successfully switching between flight mode and takeoff-landing mode at any time [Reference Li, Qiu and Zhao4, Reference Madangopal, Khan and Agrawal5] are the main constraints for existing FWMAVs during mission execution. There is an urgent need to provide a comprehensive, versatile, and highly adaptable takeoff method [Reference Xiang, Du and Li6].
Bionics is an important source of scientific and technological innovation, and learning from nature provides new principles, technologies, and methods for solving difficult scientific and engineering problems [Reference Noda, Nakata and Liu7]. In the past, the takeoff of various insects has been observed and analyzed. Houseflies (subfamily Calyptratae) can move halteres independently during takeoff, which can use the halteres to maintain takeoff stability [Reference Yarger, Jordan and Smith8]. It has also been found that the removal of halteres reduces the takeoff speed and stability of houseflies [Reference Yarger, Jordan and Smith8]. The amplitude of flapping is crucial to the average wingtip speed during the takeoff of bees. While the square of the wingtip speed is proportional to the square of air power [Reference Yang, Li and Hao9]. In addition, the average wingtip speed during takeoff causes the angle between the forewings and hindwings of bees to increase first and then decrease. It indicates that a larger wing curvature at low speeds is beneficial for increasing flapping speed [Reference Yang, Li and Hao9]. Butterflies, a hot topic in current biomimetic robot research, have significant research value for scientists in terms of the function of their wings during takeoff. The impact of couple-clipping on the takeoff performance of Pieris rapae has been investigated. It was found that couple-clipping reduces the takeoff performance of butterflies [Reference Ma, Zhao and Ma10]. Another study found that tailless butterflies adjust the peak angle of attack of the inner wing during the downstroke when turning on an incline, which can maintain an appropriate angle of tilt and sustain takeoff thrust and flight speed during the turn [Reference Dash, Parhi, Muni and Das11].
A butterfly is an excellent flying ability insect including flexible takeoff capability, outstanding flight maneuverability, stable hovering, and low flight noise [Reference Henningsson and Johansson12]. These advantages make butterfly an ideal biomimetic object for FWMAVs. The special structure and flapping mode of butterfly wings can generate efficient lift, which is crucial for their slow flight such as nectar collection [Reference Henningsson and Johansson12]. In the maneuverability, they can rapid directional changes and maneuverable flight, including flexibly navigate in complex environments and effectively evade predators [Reference Shen, Ji and Li13]. In addition, they can takeoff quickly and land slowly from various surfaces, including vertical and horizontal surfaces, even ceiling, which can enhance their adaptability in different environments [Reference Shen, Ji and Li13]. Furthermore, it has also found that the wing surface of butterfly curls into a shape of cup during flapping to increase the impulse and efficiency of the stroke [Reference Johansson and Henningsson14]. However, current research on biomimetic butterfly mainly focuses on imitating the complex structure of butterfly wings [Reference Huang, He and Zou15] and the motion mode during flight [Reference Huang, Chen and He16], as well as the muscle system of butterflies [Reference Huang, He and Zou15], while there is less research on the aerodynamics of butterfly takeoff.
In this paper, the Chinese yellow swallowtail (Papilio xuthus) was chosen as the bionic research subject. The flapping motion during the takeoff was captured and parameterized. On this basis, a biomimetic finite element aerodynamic model of P. xuthus was established, and flapping wing aerodynamics and vorticity distribution of the forewing at various angles of attack were studied. The aerodynamic behaviors of butterfly during takeoff have great significance to the design of low noise and high adaptability FWMAVs.
2. Materials and methods
2.1 Capture the takeoff motion
The takeoff motion of P. xuthus is captured by a high-speed camera (i-SPEED 3, Olympus Inc., Japan), as shown in Figure 1.
The takeoff motion capture system of P. xuthus.

Figure 1 Long description
A diagram of a takeoff motion capture system for a butterfly. The system includes a camera mounted on a tripod, a platform with a butterfly, and four LEDs positioned around the platform. The camera is directed towards the butterfly on the platform, capturing its movements. The LEDs are labeled as LED 1, LED 2, LED 3, and LED 4, and are placed at different corners of the setup to provide illumination. The platform holds the butterfly in place for observation and recording.
Five healthy adult P. xuthus with intact wings and no physical damage were selected as test specimens to ensure the reliability of takeoff motion data. Each specimen underwent 10 takeoff trials, totaling 50 trial attempts. Among these, 34 successful takeoff processes – defined as the specimen completely detaching from the test platform and finishing flight attitude adjustment – were screened for subsequent analysis, with invalid data excluded. For data processing, the valid data from 3 repeated trials of each specimen were first averaged to reduce errors caused by single-trial differences. The wingtip coordinates captured by the high-speed camera were processed frame-by-frame using i-SPEED software, followed by spline curve fitting via Origin 9.0 to eliminate random noise in the data. By calculating the mean values of the 34 successful takeoff samples, the average values and variation trends of each parameter were derived, ensuring the statistical significance of the results.
Each P. xuthus was placed on a horizontal plate to record the flapping motion during takeoff motion. As shown in Figure 1, P. xuthus was placed on a 100 × 100 mm horizontal platform. A high-speed camera with a shooting frequency of 3,000 Hz, aligned directly to the platform, was used to capture images from the side of the specimen. When the P. xuthus strops stably on the plane, the capture switch was triggered. The entire process from takeoff to off-platform was recorded. The top-left corner of the image taken by high-speed camera was set as the origin of the coordinate system, and the entire image coordinate plane was designated as the xoy plane. After data processing, the absolute coordinates of every point on P. xuthus’s wing during takeoff could be obtained.
The environmental conditions were strictly controlled, the shooting was conducted in a laboratory environment: the temperature was set at 25°C, the relative humidity was maintained at 50∼70%, the wind was controlled to a speed of ≤1.5 m/s, and the air pressure was stabilized at 1,013 hPa (standard atmospheric pressure).
2.2 3D finite element model for P. xuthus
Based on the morphological measurements of the P. xuthus (Figure 2a), the surface of P. xuthus’s wing was scanned by stereotype microscope (SteREO Discovery V20, Carl Zeiss Microimaging Inc., Germany). The structural parameters such as wingspan, chord length, contour curves, and the microstructure of the wing surface were obtained (Figure 2b). Considering the complexity of building a real 3D P. xuthus model and the computation of aerodynamic simulation, these micro-details on the wings, such as scales and microtrichia, were ignored. The overall shape of the wings, the main veins, and the variation in wing thickness from the wing root to the wing tip were focused [Reference Chen and Skote17]. After summarizing of geometry data, a finite element model of the butterfly flapping wing was established by ANSYS SCDM 2021R2, as shown in Figure 2(b). About the fluid domain, the vertical distance was the same size of the chord line of the model, the distance between the inlet boundary to the leading edge of the model was 1.5 times the chord length, and the distance between the outlet boundary to the trailing edge of the model was 4 times the chord length, as shown in Figure 2(e). In addition, P. xuthus’s forewing were meshed by ANSYS Workbench 2021R2. To improve the accuracy of the aerodynamic simulation, the boundary layer meshes of near-wall surface were set, as shown in Figure 2(f). The first layer mesh size (y+) was set to be 1% of the boundary layer thickness of the trailing edge. After meshing, the total number of elements was 3,540,000, and the number of nodes was 6,500,000. The mesh size of external flow field was set to 8.00 mm, and the mesh size of model was 0.15 mm. To guarantee the accuracy and independence of the numerical simulation results, systematic verification of mesh density and time step was conducted. Upon further mesh refinement, the relative errors of all key aerodynamic parameters are controlled within 2%, and no significant reduction in errors is observed.
(a) A real wing of P. xuthus; (b) The 3D finite element model of P. xuthus; (c) The thickness detail of the forewing; (d) The 3D model of forewing; (e) The computational domain of the forewing model; (f) internal boundary meshing diagram.

Figure 2 Long description
Panel A: A photograph of a butterfly wing with visible patterns and a scale bar indicating 10 millimeters. Panel B: A 3D finite element model of the butterfly wing, showing a detailed structure. Panel C: A close-up view of the thickness detail of the forewing, depicted as a 3D model. Panel D: An enlarged 3D model of the forewing, highlighting its surface texture. Panel E: A computational domain of the forewing model, shown as a cube with a hole in the center. Panel F: An internal boundary meshing diagram of the forewing model, displaying a detailed mesh structure.
2.3 Aerodynamics
The k-ω SST low Reynolds number (Re) turbulence equation model is selected as the turbulence model. About boundary condition, the velocity boundary was selected as the inlet boundary, and the velocity was calculated by the Re calculation formula; the pressure boundary is selected as outlet boundary.
The flapping speed of the P. xuthus was set as 4 m/s [Reference Ortega, Eastwood, Vogt and Ithier18]. Its forewing average chord length is 31.18 mm by measuring. So, the Re can be calculated by Re formula,
 \begin{equation}Re=\frac{\rho _{a}\nu c_{L}}{\mu }\end{equation}
where v is the flapping velocity of P. xuthus, 4 m/s, ρ is the air density: 1.225 kg/m3, C L is the average chord length: 31.18 mm, and μ is the air viscosity: 1.789 × 10⁻⁵ kg/m·s. After calculating, the Re of the model during flapping is 8.491 × 10³, which belongs to the low Re range.
3. Results and discussion
3.1 Takeoff motion capture
Each P. xuthus was tested three times, and the image sequence that best shows the P. xuthus motion trajectory was selected. The tips of the left and right wings of the P. Xuthus in each image were marked, and the x and y coordinates of the marked wing tips were exported to origin to provide a data foundation for curve fitting.
In Figure 3, the flapping motion of P. xuthus was observed to be strongly symmetrical, with 34 successful takeoffs out of 50 experimental attempts. The takeoff process can be divided into four stages. First stage is the preparation (t = 241ms), where P. Xuthus remains stationary on the plate with wings kept flat (Figure 3(a)). Second stage is the initiation (t = 323 ms to t = 550 ms), during which P. xuthus begin to flap. Due to the limitations of the platform, the amplitude of flap is small (Figure 3(c)). During the downstroke, the foreleg and midleg start to extend and leave the platform (Figure 3(d)). Its body is gradually lifted, forming an angle of about 70°with the platform (Figure 3(e)). Third stage is the disengagement (t = 583 ms to t = 703 ms), where the hind legs of P. xuthus detach from the platform (Figure 3(g)), with the wingbeat frequency doubles. The last stage is the adjustment (t = 778 ms to t = 910 ms). After leaving the platform, P. xuthus experiences a brief descent to adjust its flight posture (Figure 3(i)), then its body axis aligns horizontally (Figure 3(k)). It begins to fly until the adjustment stage is completed (Figure 3(l)). Throughout the process of takeoff, the butterfly always maintains a line from the wingtips to the wing base perpendicular to the body axis to keep its wingspan at the maximum value.
The video sequence captured of P. xuthus dynamically during takeoff.

Figure 3 Long description
Panel A: A butterfly is positioned on a platform with its wings slightly raised. Panel B: The butterfly's wings are more elevated, preparing for takeoff. Panel C: The butterfly's wings are fully extended, ready to flap. Panel D: The butterfly begins to lift off from the platform. Panel E: The butterfly is mid-flight, moving upward. Panel F: The butterfly continues to ascend. Panel G: The butterfly is higher in the air, moving away from the platform. Panel H: The butterfly is further away, still in flight. Panel I: The butterfly is nearly out of the frame, continuing its flight. Panel J: The butterfly is almost out of sight, having completed its takeoff. Panel K: The butterfly is barely visible, indicating it has flown away. Panel L: The platform is empty, with no butterfly in sight.
3.2 Wingtip trajectory and flapping kinematics
The wingtip motion of P. xuthus during takeoff was captured by high-speed camera. The video was processed frame by frame by i-SPEED. The positions of the left and right wingtips were marked in every frame to obtain the coordinates of the wingtips in every frame. Subsequently, the scale was calculated to determine the actual coordinates of the wingtips in every frame. The coordinates of the wingtips were imported into Origin 9.0. After spline curve fitting, the motion trajectories of the wingtips of P. xuthus’s forewings were ultimately obtained, as shown in Figure 4.
Wingtip trajectories of P. xuthus during takeoff. The wingtips move from the red point in the lower right corner to the dark blue area in the upper left corner (Solid lines represent the left wingtip, and dashed lines represent the right wingtip).

Figure 4 Long description
A line graph titled Wingtip_Curve displays the trajectories of the left and right wingtips during takeoff. The horizontal axis is labeled X(Pixel)/mm and ranges from 50 to 600. The vertical axis is labeled Y(Pixel)/mm and ranges from 500 to 750. The graph includes a color bar indicating time progression from red to blue. The solid lines represent the left wingtip, starting from the lower right corner in red and moving to the upper left corner in dark blue. The dashed lines represent the right wingtip, following a similar trajectory. Both wingtips show a downward trend as they move from right to left.
By comparing the wingtip trajectory curves of P. xuthus, it can be observed that during the takeoff, it starts from the lower right corner of the image and gradually flies toward the upper left corner. Comparing the trajectories of the left and right wingtips, it is observed that although the right wingtip is generally higher than the left, the difference in height remains relatively constant. Also, the trajectories are essentially the same. That indicates that the amplitude of movement for both wings is roughly the same, which matches the symmetry of the P. xuthus’s takeoff process. During the preparation stage (Figure 3(a)), its body axis is in a horizontal position, and the amplitude of the wingtip trajectory changes slowly, approximately forming a vertical straight line. In the initiation stage (Figure 3(b)–3(e)), due to the limitations of the platform, it is adjusting its posture that the front-middle part of its body is gradually lifted until the body axis is at an angle of about 70°with the platform. The wingtip trajectory forms a curve with a small curvature. In the detachment stage (Figure 3(f)–3(h)), the amplitude of the wingtip trajectory changes rapidly and is approximately a straight line. The frequency of flap increased. In this time, P. xuthus’s posture has been adjusted, and it is beginning to detach from the platform. In the adjustment stage (Figure 3(i)–3(l)), the speed of amplitude change in the wingtip trajectory decreases, and it forms a curve with a large curvature. Its posture is changed, and its body axis is once again in a horizontal position.
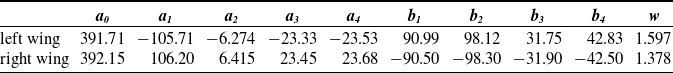
Coefficients of the first four Fourier series terms in the curve fits.

Table 1 Long description
A table comparing the coefficients of the first four Fourier series terms in the curve fits for the left and right wings. The table has 2 rows and 11 columns. The columns are labeled as a 0, a 1, a 2, a 3, a 4, b 1, b 2, b 3, b 4, and w. The row labels are left wing and right wing. Row 1: left wing, 391.71, 105.71, 6.274, 23.33, 23.53, 90.99, 98.12, 31.75, 42.83, 1.597. Row 2: right wing, 392.15, 106.20, 6.415, 23.45, 23.68, 90.50, 98.30, 31.90, 42.50, 1.378.
To obtain the equations of the takeoff motion curves, the absolute coordinates of the wingtips of P. xuthus obtained from Figure 4 were imported into the Matlab R2022a the fourth-order Fourier series is used to complete the curve fitting, and the fitting equation of the left and right wing tip trajectories is obtained. The coefficient parameters of the first four Fourier series terms in the curve are shown in Table 1.
-
• The left wing: f(x) = a0 + a1*cos(x*w) + b1*sin(x*w) + a2*cos(2*x*w) + b2*sin(2*x*w) + a3*cos(3*x*w) + b3*sin(3*x*w) + a4*cos(4*x*w) + b4*sin(4*x*w)
-
• The right wing: f(x) = a0 + a1*cos(x*w) + b1*sin(x*w) + a2*cos(2*x*w) + b2*sin(2*x*w) + a3*cos(3*x*w) + b3*sin(3*x*w) + a4*cos(4*x*w) + b4*sin(4*x*w)
3.3 Aerodynamic characteristic analysis
The trajectory function set for the butterfly forewing tip, obtained in the previous section 3.2, is imported as a UDF file into Ansys Fluent 2021R2 to simulate the aerodynamic performance during the forewing’s transient takeoff motion. The results are presented in Figure 5.
(a) The flapping stage diagram of the takeoff motion; (b) The diagram of the flapping amplitude of the forewing of P. xuthus during takeoff with time; (c) The lift coefficient diagram of the forewing; (d) The drag coefficient diagram of the forewing; (e) The diagram of the average aerodynamics with the angle of attack.

Figure 5 Long description
Panel A: A diagram showing the flapping stages of the takeoff motion, labeled from I to VII, with angles ranging from -90 degrees to 0 degrees. Panel B: A line graph depicting the flapping amplitude of the forewing of P. xuthus during takeoff over time, with the horizontal axis labeled 'Time / s' and the vertical axis labeled 'Displacement / mm'. The graph includes two lines representing the left and right wings. Panel C: A line graph showing the lift coefficient of the forewing over time, with the horizontal axis labeled 'Time / s' and the vertical axis labeled 'Lift coefficient'. The graph includes multiple lines representing different angles of attack. Panel D: A line graph displaying the drag coefficient of the forewing over time, with the horizontal axis labeled 'Time / s' and the vertical axis labeled 'Drag coefficient'. The graph includes multiple lines representing different angles of attack. Panel E: A line graph illustrating the average aerodynamics with the angle of attack, with the horizontal axis labeled 'Angle of attack' and the vertical axis labeled 'Average aerodynamics'. The graph includes multiple lines representing different aerodynamic coefficients.
From Figure 5(a and b), the entire process can be divided into two cycles (T = 0.22 s), each cycle can be divided into seven stages (Figure 5(a), including: the forewing flaps upward from 0° to −90° (I, t = 0.22 s to t = 0.26 s); flaps downward from −90° to 90° (II, t = 0.26 s to t = 0.30 s); flaps upward from 90° to −90° (III, t = 0.30 s to t = 0.33 s); flaps downward from −90° to 90° (IV, t = 0.33 s to t = 0.36 s); flaps from 90°to 0° (V, t = 0.36 s to t = 0.37 s); flaps from 0° to 90° (VI, t = 0.37 s to t = 0.41 s); and flaps from 90° to 0° (VII, t = 0.41 s to t = 0.44 s).
Figures 5(c, d, and e) are the curves of lift coefficient, drag coefficient, and average aerodynamics of the forewing of P. xuthus at Re = 8.49 × 10³. From Figure 5(c), it can be seen that the variation trend of the lift coefficient of the forewing of P. xuthus is basically consistent within first cycle (t = 0.22 s to t = 0.44 s), when the angle of attack is less than 20°. When the angle of attack is 30°, the variation amplitude of its forewing lift coefficient is not significant, and the amplitude is the smallest. It indicates that at this time, the forewing of P. xuthus has experienced stall [Reference Sun19]. In step I, the lift coefficient shows a decreasing trend from 0.22 s to 0.26 s when the angle of attack is less than 20°. The minimum value appears at 0.26 s. From the flapping amplitude diagram (Figure 5b), it can be seen that the lift coefficient shows a minimum value when the forewing flaps from upward to downward (t = 0.26 s). In step II, the lift coefficient of the forewing shows an increasing trend, which is about twice that of the previous stage’s decrease. In step III, its lift coefficient shows a decreasing trend, which is basically consistent with the increase in step II. In step IV, it is the same as step II. In step V, it is exactly the opposite of step I. In step VI, its lift coefficient shows a decreasing trend, which is the same as step V. In step VII, this is the last stage of a cycle, and its lift coefficient shows a decreasing trend, eventually decreasing to the same as the beginning of step I. At this point, a cycle ends. The results show that during the takeoff, when the forewing flaps upward, its lift coefficient will gradually decrease, while when it flaps downward, its lift coefficient will gradually increase. The extreme values of lift coefficient will be shown when the forewing changes the direction of flapping. The minimum value will appear when it flaps from upward to downward. On the opposite, the maximum value will appear when it flaps from downward to upward. In addition, when the angle of attack is less than 20°, the lift coefficient of the forewing shows a trend of increasing first and then decreasing with the increase of the angle of attack [Reference Molaa and Abdulwahid20, Reference Zhu, Sun and Wang21]. When the angle of attack is 10°, the lift coefficient of the forewing reaches its maximum value, which is 72.00% higher than 5° angle of attack, and 59.26% higher than 20° angle of attack. This may be due to the fact that when the angle of attack increases from 5° to 10°, the airflow path on the upper surface of the forewing becomes longer, while the airflow path on the lower surface is relatively shorter. And the airflow speed on the upper surface of the forewing increases, the pressure decreases. While on the lower surface, the speed decreases, the pressure increases, so the lift coefficient rises [Reference Liu and Aono22]. When the angle of attack increases from 10° to 20°, the critical angle of attack is gradually approached, the airflow on the upper surface of the forewing will separate in advance, forming vortices, which leads to a sharp decrease in lift coefficient [Reference Hu, Wang, Zhang and Zhang23].
From Figure 5(d), it can be seen that the variation trend of the drag coefficient of the forewing of P. xuthus is basically consistent within a cycle when the angle of attack is less than 20°. When the angle of attack is 30°, its drag coefficient shows an opposite variation trend to the drag coefficients of the other three angles of attack. For example, in the I step, the drag coefficients of the first three angles of attack show an increasing trend, while the drag coefficient of the 30° angle of attack shows a decreasing trend. The maximum value of the drag coefficients of the first three angles of attack is reached at 0.26 s, while the minimum is reached at the 30° angle of attack. It indicates that during the takeoff, when the drag coefficient of the forewing will increase when it flaps upward. And that will decrease when it flaps downward. The extreme values of drag coefficient will be shown when the forewing changes the direction of flapping. The maximum value will appear when it flaps from upward to downward, while the minimum value will appear when it flaps from downward to upward. In addition, it can also be seen that the drag coefficient of the forewing shows a trend of increasing first and then decreasing with the increase of the angle of attack when the angle of attack is less than 20°. The maximum value of the drag coefficient is reached when the angle of attack is 10°, which is 2.6 times higher than 5° angle of attack, and 38.46% higher than 20° angle of attack.
From Figure 5(e), it can be seen that the average lift coefficient, average drag coefficient, and average lift-drag ratio of the forewing of P. xuthus all show a trend of increasing first and then decreasing during takeoff. The increase and decrease of the average lift coefficient are both greater than those of the average drag coefficient. This result is consistent with the variation range of lift and drag coefficients between 5° and 30° angles of attack obtained in Figures 5(c and d). It indicates that the average lift-drag ratio of forewing increases first and then decreases with the increase of the angle of attack. In addition. When the angle of attack is 14°, the maximum value of the average lift coefficient is reached. While the maximum value of average drag coefficient is reached when the angle of attack is 10°. their minimum values are both reached at 30°. And when the angle of attack is 20°, the highest lift-drag ratio of the forewing appears. Its maximum value is 8.2 times higher than 5° angle of attack, 61.40% higher than 10° angle of attack, and 55.93% higher than 30° angle of attack.
In addition, the difference between the optimal angle of attack for lift coefficient (14°) and that for lift-drag ratio (20°) is mainly due to the distinct sensitivities of different aerodynamic performance metrics to the angle of attack (AoA). This is mainly because different aerodynamic performance metrics have distinct sensitivities to the angle of attack (AoA). Specifically, the maximum lift coefficient at a 10° angle of attack stems from the optimal pressure differential between the upper and lower surfaces of the forewing: at this angle of attack, airflow remains fully attached to the forewing surface without premature separation, creating the maximum pressure gradient and thus yielding the peak lift. In contrast, the maximum lift-to-drag (L/D) ratio at a 20° angle of attack is driven by a superior balance between lift generation and drag attenuation. As the angle of attack increases from 10° to 20°, the lift coefficient experiences a moderate decrease due to incipient mild airflow separation, while the drag coefficient declines far more significantly – this is attributable to the stable attachment of leading and trailing edge vortices (LEV/TEV) on the forewing’s upper surface and a concomitant reduction in vortex shedding. This asymmetric variation in lift and drag ultimately results in the highest aerodynamic efficiency (L/D ratio) at a 20° angle of attack. So, this indicates that the aerodynamic efficiency in flight is the optimal at the 20° angle of attack.
From Figures 5(b and c), it can be seen that the aerodynamic efficiency is the highest at 20° angle of attack during takeoff of P. xuthus. So, the vorticity characteristics at 20° angle of attack are analyzed. To simplify the calculation, the flapping cycle can be divided into four stages: the first stage is from 0° to −90°, the second stage is from −90° to 90°, the third stage is from 90° to −90°, and the fourth stage is from −90° to 0°.
From Figure 6(a), when the forewing is at the first stage (T = 0.22 s to T = 0.26 s), the leading-edge vortex (LEV) and the trailing edge vortex (TEV) begin to grow at the leading and trailing edges, respectively, after the residual vortex flow leaves the upper surface [Reference Zou, Lai and Yang24]. The direction is from the upper surface to the lower surface of the forewing (Figure 6(b)). This results in the formation of a low-pressure area on the lower surface of the forewing and the reduction of the pressure difference between the upper and lower surfaces, which thereby cause the lift coefficient of the forewing to decrease to −0.3 [Reference Hu, Wang, Zhang and Zhang23–Reference Pullin and Wang25]. Also, both LEV and TEV remain attached to the lower surface throughout the upstroke (Figure 6(c)). During this stage, the lift coefficient of the forewing continues to decrease. When the forewing is at the horizontal position, the LEV and TEV are at their largest scale [Reference Yarger, Jordan and Smith8] (Figure 6(a)). This matches the trend of the lift coefficient change from 0.22 s to 0.26 s at a 10° angle of attack in Figure 5(b). In addition, the structure of LEV and TEV is not stable, so they will shed during the upstroke, which causes the drag coefficient of the forewing to increase to 0.15 [Reference Hu, Wang, Zhang and Zhang23]. This matches the trend of the drag coefficient change from 0.22 s to 0.26 s at a 10° angle of attack in Figure 5(c). When the forewing is at the second stage (T = 0.27 s to T = 0.30 s), it can be observed that most of the LEV and TEV on the lower surface of the forewing have shed (Figure 6(d)), while the LEV and TEV on the upper surface develop rapidly and attach to the upper surface (Figure 6(e)), which forms a low-pressure area on the upper surface. It creates a significant pressure difference between the upper and lower surfaces, which causes the lift coefficient of the forewing to continue to increase to 0.43 [Reference Zou, Lai and Yang24, Reference Pullin and Wang25]. This matches the trend of the lift coefficient change from 0.26 s to 0.30 s at a 10° angle of attack in Figure 5(b). During this stage, the structure of LEV and TEV is more stable, and the shedding phenomenon is reduced (Figure 6(f)). Therefore, the drag coefficient of the forewing is reduced to 0.025 [Reference Hu, Wang, Zhang and Zhang23]. This matches the trend of the drag coefficient change from 0.26 s to 0.30 s at a 10° angle of attack in Figure 5(c). When the forewing is at the third stage (T = 0.31 s to T = 0.33 s), the distribution of LEV and TEV is essentially the same as the first stage. When the forewing is at the fourth stage (T = 0.37 s to T = 0.41 s), the distribution of LEV and TEV is essentially consistent with the second stage. In summary, the vortex wake patterns of the forewing of P. xuthus during the takeoff can be consistently matched with the time curves of aerodynamic forces.
Vorticity diagram of the forewing of P. xuthus during takeoff. (a–c) The first stage (0° to −90°); (d–f) The second stage (−90° to 90°); (g–i) the third stage (90° to −90°); (j–l) The fourth stage (−90° to 0°).

Figure 6 Long description
A vorticity diagram of the forewing of P. xuthus during takeoff. Panel A: Vorticity diagram at T = 0.22s showing leading-edge vortex (LEV) and trailing-edge vortex (TEV). Panel B: Vorticity diagram at T = 0.24s showing LEV and TEV. Panel C: Vorticity diagram at T = 0.26s showing LEV and TEV. Panel D: Vorticity diagram at T = 0.27s showing LEV and TEV. Panel E: Vorticity diagram at T = 0.28s showing LEV and TEV. Panel F: Vorticity diagram at T = 0.30s showing LEV and TEV. Panel G: Vorticity diagram at T = 0.31s showing LEV and TEV. Panel H: Vorticity diagram at T = 0.32s showing LEV and TEV. Panel I: Vorticity diagram at T = 0.33s showing LEV and TEV. Panel J: Vorticity diagram at T = 0.37s showing LEV and TEV. Panel K: Vorticity diagram at T = 0.39s showing LEV and TEV. Panel L: Vorticity diagram at T = 0.41s showing LEV and TEV.
In addition, the high-speed camera recordings captured the deformation and motion of the forewings during takeoff (Figure 3). By correlating the simulated instantaneous vorticity fields (Figure 6) with the wing motion phases, it can be observed that the formation and shedding of the LEV and the trailing-edge vortex in the CFD results align well with the wake patterns inferred from the video sequences. Although the video does not provide quantitative flow field data, the qualitative consistency supports the credibility of the simulated flow structures.
So, the obtained optimal angle of attack and vorticity parameters can provide new design ideas for solving problems such as insufficient takeoff capability and difficult mode switching of FWMAV design.
4. Conclusion
In this paper, P. xuthus is selected as a research object, and its takeoff motion was captured by the high-speed camera system. The flapping trajectory of the forewings was obtained. During the takeoff, the forewings of P. xuthus have strong symmetry and flapping frequency increases gradually. Its foreleg and midleg are extended to increase the angle between the body axis and the horizontal plane and alter the angle of attack of the forewings to generate sufficient lift to complete takeoff. In addition, the line from the wingtip to the body center of the forewing of P. xuthus is perpendicular to the body axis all the time.
After that, a three-dimensional finite element model of the forewing is established. The aerodynamic characteristics during the takeoff are analyzed. The results show that when the angle of attack is between 0° and 20°, the lift coefficient, drag coefficient, and average lift-to-drag ratio of the forewing of P. xuthus all exhibit a trend of increasing first and then decreasing as the angle of attack increases. In the vorticity characteristics analysis, when the forewing of P. xuthus flaps upward, the LEV and TEV begin to grow at the leading and trailing edges. Respectively, after the residual vortex flow leaves the upper surface, a low-pressure area is formed on the lower surface of the forewing, and the pressure difference between the upper and lower surfaces is reduced. This causes the lift coefficient of the forewing to decrease. Both LEV and TEV remain attached to the lower surface and extend during the upstroke, which can continuously reduce the lift coefficient of the forewing. However, the structure of LEV and TEV is not stable and gradually sheds during the upstroke. This increases the drag coefficient of the forewing. When the forewing flaps downward, the LEV and TEV on the lower surface have already shed, while the LEV and TEV on the upper surface develop rapidly and attach to the upper surface. A low-pressure area is created on the upper surface and a significant pressure difference between the upper and lower surfaces is caused. This leads to a continuous increase in the lift coefficient of the forewing. During this process, the structure of LEV and TEV remains stable, and the flow separation is reduced. Therefore, the drag coefficient of the forewing is lowered. This basic investigation will be beneficial for understanding the takeoff mode of P. xuthus.
This study focuses on the flapping takeoff trajectory and aerodynamic characteristics of P. xuthus. Future research can be extended in two key aspects: expanding the research scope and optimizing methodologies. About research objects, the limitation of relying on a single species can be addressed by incorporating other lepidopteran insects, such as the small white butterfly (Pieris rapae) and skippers (Hesperiidae). By comparing the flapping patterns and motion data across these species, the common principles and species-specific traits of insect flapping motion can be systematically identified. About optimizing methodologies, the current Fourier fitting approach does not account for the influence of environmental airflow disturbances (e.g., gentle breezes, turbulence) on wingtip trajectories. In subsequent work, wind tunnel experiments can be integrated to develop a coupled model of “airflow disturbance-flapping attitude adjustment,” which will further improve the adaptability of motion fitting results to complex real-world environments.
Data availability statement
The data that support the findings of this study are available from the corresponding author upon reasonable request.
Author contribution
The study conception was designed by C. Liu. Material preparation, data collection and analysis were performed by C. Liu, C.Y. Zhu and H.M. Wu. The first draft of the manuscript was written by C.Y. Zhu, H.M. Wu and Y.M. Wang. The manuscript was revised by L.N. Sun, Z.J. Jiang and G.D. Chen. And all authors commented on the early versions of the manuscript.
Funding statement
This work was supported by the National Natural Science Foundation of China (grant numbers 52305321); The Natural Science Foundation of Jiangsu Province (BK20230496); China Postdoctoral Science Foundation Funded Project (2023M732536 and 2024T170630); Jiangsu Province Excellence Postdoctoral Program (2023ZB218); The National Key R&D Program of China (2022YFB4702202); The Jiangsu Provincial Key Technology R&D Program (BE2021009-02).
Competing interests
The authors declare no conflicts of interest.