Introduction
Vertebrate hosts commonly harbour concurrent infections of helminths which may interact with one another in the same site within the host in either synergistic, antagonistic or negligible ways (Christensen et al., Reference Christensen, Nansen, Fagbemi and Monrad1987; Cox, Reference Cox2001; Poulin, Reference Poulin2001). Interactions between helminths that occupy different sites within a host are more poorly studied and have mainly focused on mammalian hosts, where both synergistic and antagonistic interactions occur (Christensen et al., Reference Christensen, Nansen, Fagbemi and Monrad1987; Curry et al., Reference Curry, Else, Jones, Bancroft, Grencis and Dunne1995; Corrêa-Oliveira et al., Reference Corrêa-Oliveira, Golgher, Guilherme, Carvalho, Massara, Caldas, Colley and Gazzinelli2002). Studies on indirect interactions between concurrent helminth infections in fish are rare, especially under field conditions. Nevertheless, available evidence would suggest that larval cestodes demonstrate the greatest potential to influence indirectly the occurrence of other helminth species in concurrent infections (Markov & Kosareva, Reference Markov and Kosareva1962; Zhokhov & Pugacheva, Reference Zhokhov and Pugacheva2012; Morley & Lewis, Reference Morley and Lewis2017). The occurrence of intestinal helminths in fish has been shown to be indirectly affected by co-infection with plerocercoids of the cestode Triaenophorus nodulosus that reside in the liver of perch (Perca fluviatilis). These plerocercoids appear to induce a variable effect on such parasites, resulting in a significant reduction in the prevalence of acanthocephalans and nematodes, but inducing no effect on the occurrence of cestodes and trematodes, in the digestive tract (Morley & Lewis, Reference Morley and Lewis2017). Furthermore, the distribution of the trematode Bunodera lucioperca along the length of the intestine may also be altered in T. nodulosus-infected perch (Izvekova & Tyutin, Reference Izvekova and Tyutin2014). Such effects on intestinal helminths may be due to either cestode-induced damage to the liver, the release of parasite excretory/secretory (E/S) products, or the host's immune response (Morley & Lewis, Reference Morley and Lewis2017).
Similarly, larval cestodes occupying other sites within the fish host may also indirectly affect the occurrence of intestinal helminths. The peritoneal (body) cavity of fish can harbour the plerocercoid stage of a number of different cestode species (Dubinina, Reference Dubinina1980; Williams & Jones, Reference Williams and Jones1994; Scholz & Kuchta, Reference Scholz and Kuchta2016). One of the most extensively studied species is Ligula intestinalis, which infects a range of freshwater cyprinid fish (Dubinina, Reference Dubinina1980). Infections with L. intestinalis (ligulosis) can cause extensive pathology, resulting in gross effects on the body, altered physiology, organs and blood composition, with the most significant impact being the inhibition of host reproduction induced by parasite E/S products (Hoole, Reference Hoole, Pike and Lewis1994; Hoole et al., Reference Hoole, Carter and Dufour2010). The impact of this larval cestode on intestinal helminths has been found to be highly variable, demonstrating in barbel (Labeobarbus crassibarbis) synergism with the caryophyllidean cestode Khawia sp. (Zhokhov & Pugacheva, Reference Zhokhov and Pugacheva2012), and in bream (Abramis brama) antagonism with Caryophyllaeus laticeps (Markov & Kosareva, Reference Markov and Kosareva1962). However, potential indirect effects of L. intestinalis on helminths residing in other host organs, such as in the eye, remain unknown.
Infections of the eyes of fish with trematode metacercariae are common in freshwater habitats, transmission being attributed largely to the wide distribution of piscivorous avian definitive hosts. Over a large scale, fish acquire infections after casual contact with free-living cercariae, which emerge in large numbers from freshwater snail intermediate hosts. Cercariae actively penetrate fish before migrating to the eye to form metacercariae (Haas, Reference Haas2003; Haas et al., Reference Haas, Wulff, Grabe, Meyer and Haeberlein2007) and eyeflukes are capable of causing extensive pathology to the eyes in heavy infections. Under certain circumstances, metacercariae demonstrate bilateral asymmetry in their distribution between left and right eyes of individual fish (Rau et al., Reference Rau, Gordon and Curtis1979; Graczyk, Reference Graczyk1991; Wayland & Chubb, Reference Wayland and Chubb2016), a phenomenon that may function as a means to mitigate the impact of infection on the host (Johnson et al., Reference Johnson, Koprivnikar, Orlofske, Melbourne and Lafonte2014). However, mechanisms that cause asymmetry are not fully understood and may potentially be indirectly influenced by the occurrence of other helminths, such as L. intestinalis, in the host.
Experimental studies on the related species Schistocephalus solidus in the three-spined stickleback (Gasterosteus aculeatus) provide some important pointers and likely indirect influences on other helminths in ligulosed fish. Laboratory exposure of fish harbouring S. solidus to cercariae of the eyefluke Diplostomum pseudospathaceum showed that only those sticklebacks harbouring a specific ‘high-growth’ strain of this cestode resulted in higher abundance of metacercariae in the eyes compared with S. solidus non-infected controls. A follow-up, field-based experiment using caged S. solidus-infected sticklebacks placed in the littoral zone of a lake found that fish had a higher abundance of D. pseudospathaceum but a lower abundance of another eyefluke, Apatemon cobitidis. Furthermore, within the intestine of these fish there was a lower abundance of the trematode Sphaerostomum globiporum and a higher abundance of the cestode Proteocephalus filicollis (Benesh & Kalbe, Reference Benesh and Kalbe2016). However, these experimental results need to be treated with some caution in view of the limitations of using caged animals in the field for determining parasite transmission success. By unnaturally restricting the free movement of fish hosts, there is an elevated risk of producing false-positive or false-negative results. This is particularly important in fish infected with larval cestodes where there is extensive evidence of altered host behaviour (Dubinina, Reference Dubinina1980; Giles, Reference Giles1987; Barber & Scharsack, Reference Barber and Scharsack2010), leading to changes in spatial and temporal distribution of fish hosts in habitats (Loot et al., Reference Loot, Brosse, Lek and Guégan2001). This may, in turn, influence not only contact with free-living stages and/or infected intermediate hosts, but also the subsequent likelihood of fish becoming infected. Consequently, the experimental studies undertaken by Benesh & Kalbe (Reference Benesh and Kalbe2016) would benefit from complementary studies under field conditions, to determine if such phenomena occur naturally. The present study, using an existing dataset, will examine the natural influence of L. intestinalis on the occurrence and bilateral asymmetry of eyeflukes in the roach, Rutilus rutilus, a common freshwater fish from a lake site in south-east England.
Materials and methods
Fish sampling was undertaken at Dinton Pastures Country Park, near Reading in south-east England (GPS coordinates 51.443128, −0.883560). The park was opened in 1979 on a site previously exploited for gravel extraction. Eight gravel-pit lakes of various sizes were constructed within the original extracted site to provide an environment suitable for both wildlife and recreational needs, particularly water sports and fishing. Sampling of roach was undertaken in one of the aquatic habitats, namely White Swan Lake, which is a 24-acre elongated lake orientated on a north–south axis and used exclusively for coarse fishing, including carp, rudd and roach. A sample of 323 roach were seine-netted during the month of September 2002 and immediately transferred to the laboratory for investigation. The total body length and weight of fresh fish were recorded before they were dissected and examined for helminths using standard parasitological techniques. The condition coefficient (K) for each individual fish was calculated as follows:
 $$K = (\hbox{body weight}/\hbox{body length}^3) \times 100.$$
Data analysis
The prevalence, mean intensity and mean abundance of eyeflukes in ligulosed and non-ligulosed roach populations were calculated according to Bush et al. (Reference Bush, Lafferty, Lotz and Shostak1997) and analysed using Quantitative Parasitology 3.0 statistical package (Reiczigel & Rozsa, Reference Reiczigel and Rozsa2005). Additional analysis was undertaken to eliminate the alternative possibility that eyefluke pathology may increase the susceptibility of roach to L. intestinalis. As many hosts harboured mixed infections of eyeflukes, these parasites were considered only collectively and the infection parameters of L. intestinalis between eyefluke-infected and non-infected roach were analysed in a similar manner.
Other analyses were undertaken using SPSS version 21 statistical package (SPSS Inc., Chicago, Illinois, USA) with one-way analysis of variance (ANOVA) used to compare K values between ligulosed and non-ligulosed fish. For analysis of any direct interactions between the occurrence of species of eyefluke within individual ligulosed and non-ligulosed fish, data were normalized by sine transformation and, following removal of zeros (fish not infected by any parasite species), analysed by linear regression. Analysis of eyefluke bilateral asymmetry was undertaken using the software tool ‘Analysis of symmetry of parasitic infections’ (http://wayland.shinyapps.io/aspi) as described by Wayland & Chubb (Reference Wayland and Chubb2016). As the present dataset contained zero counts, replicated G-tests of goodness-of-fit were not applicable and hence exact binomial tests were used to test for bilateral asymmetry with this software package.
Results
The roach population in White Swan Lake harboured an infection of L. intestinalis plerocercoids with a prevalence of 11.5% and a mean intensity of 1.44 in the peritoneal cavity of each infected fish. Comparisons of the condition of ligulosed and non-ligulosed roach (table 1) showed that there were no significant differences in length and weight of fish between the two populations (one-way ANOVA: P = 0.162, F = 1.981 and P = 0.917, F = 0.011, respectively). However, ligulosed roach did have a significantly higher K value than non-ligulosed fish (one-way ANOVA: P = 0.044, F = 4.088).
The body length (cm), weight (g) and condition (K) of ligulosed and non-ligulosed roach from White Swan Lake.

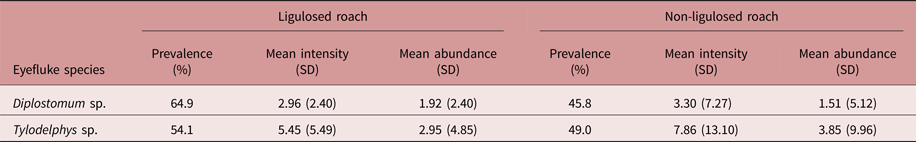
Eyeflukes were the most common helminths occurring in the roach population and these comprised two species, Diplostomum sp., occurring exclusively in the lens, and Tylodelphys sp., found only in the vitreous humour. Infections with other metazoan parasites were limited, with only the adult cestode C. laticeps occurring in the intestine of 1.4% of non-ligulosed and 2.8% of ligulosed roach. Analysis of the two eyefluke species between ligulosed and non-ligulosed fish (table 2) showed that the prevalence of Diplostomum sp. was significantly increased in ligulosed roach (P = 0.029, χ2 = 4.769) but intensity and mean abundance were unaffected (P = 0.703, t = −0.423 and P = 0.434, t = 0.819, respectively). In contrast, the occurrence of Tylodelphys sp. remained unaffected by the presence of L. intestinalis, with no significant changes in the prevalence, intensity or mean abundance (P = 0.559, χ2 = 0.341; P = 0.378, t = 0.909 and P = 0.379, t = −0.909, respectively). The alternative analysis of the occurrence of L. intestinalis between eyefluke-infected and non-infected roach demonstrated that the pathology induced by these trematodes on the host did not affect either prevalence, intensity or mean abundance of the larval cestode in the host (P = 0.356, χ2 = 0.853; P = 0.852, t = −0.178 and P = 0.502, t = 0.680, respectively).
Levels of infection of the eyeflukes Diplostomum sp. and Tylodelphys sp. in ligulosed and non-ligulosed roach from White Swan Lake.

Analysis of direct interactions between the occurrence of the eyefluke species showed that in non-ligulosed roach no significant difference in prevalence existed between the two species (P = 0.451, χ2 = 0.568) but significant differences occurred in the mean intensity and abundance (P < 0.0001, t = 3.573 and P = 0.0025, t = 3.520, respectively). However, in ligulosed fish there were no significant differences in any measure of infection (prevalence P = 0.344, χ2 = 0.897; intensity P = 0.0805, t = 1.884; mean abundance P = 0.236, t = 1.155). Further analysis of any specific relationship in individual fish between the occurrence of the two eyefluke species showed that there were no significant interactions between Diplostomum sp. and Tylodelphys sp. in either non-ligulosed (linear regression r 2 = 0 no correlation, F = 0.01, P = 0.907) or ligulosed fish (linear regression r 2 = 0.01 positive correlation, F = 0.268, P = 0.609).
Analyses of bilateral asymmetry of eyeflukes showed that infections with Diplostomum sp. demonstrated no significant asymmetry between left and right eye in either ligulosed (Exact binomial test P = 0.11) or non-ligulosed fish (Exact binomial test P = 0.18). In contrast, Tylodelphys sp. in non-ligulosed roach harboured a metacercarial burden of 537 in the left eye and 633 in the right eye. Six asymmetrical infections showed a left bias in four and a right bias in two eyes, therefore indicating an overall significant asymmetry (Exact binomial test P = 0.01). However, in ligulosed roach, Tylodelphys sp. showed no evidence of a significant asymmetry, with metacercariae being relatively evenly distributed between left and right eyes (Exact binomial test P = 0.76).
Discussion
Infections of roach with L. intestinalis plerocercoids represented only a modest proportion (11.5%) of the sampled population from White Swan Lake. However, the occurrence of L. intestinalis in fish populations is patchy, although when present may potentially achieve prevalence levels of between 70 and 90% (Sweeting, Reference Sweeting1977; Kennedy et al., Reference Kennedy, Shears and Shears2001; Zhokhov & Pugacheva, Reference Zhokhov and Pugacheva2012), thereby indicating the substantial potential of this cestode to indirectly influence the occurrence of other helminth species in habitats harbouring infected hosts. In the present study these plerocercoids appear capable of influencing the concurrent occurrence of eyeflukes in roach. Species of Diplostomum and Tylodelphys metacercariae are common parasites of the eyes of wild freshwater fish in the UK (Kennedy, Reference Kennedy1974). Several congenic species of Diplostomum and Tylodelphys, which are difficult to differentiate morphologically at the metacercarial stage, may occur in the eyes of European freshwater fish (Chappell, Reference Chappell1995). However, concurrent sampling of snails from White Swan Lake found that only two species of furcocercariae were present (Morley, unpubl. obs.). As this cercarial morphotype corresponds with those species that infect fish eyes (Blair, Reference Blair1977) it appears unlikely that numerous eyefluke species are present in this habitat.
Eyeflukes show seasonal patterns of infection, with abundance generally increasing through the summer and autumn months (Chubb, Reference Chubb1979; Chappell et al., Reference Chappell, Hardie, Secombes, Pike and Lewis1994). Sampling in the present study occurred in September, when parasite numbers tend to peak. Nevertheless, metacercarial survival in the eyes of fish is variable, e.g. Diplostomum spp. have been reported to live up to 4 years in roach (Shigin, Reference Shigin1964), whereas survival of Tylodelphys spp. can be much shorter and occasionally no more than a season in duration (Burrough, Reference Burrough1978).
The present study has shown that prevalence, but not intensity or mean abundance, of Diplostomum sp. is significantly higher in ligulosed roach, while the occurrence of Tylodelphys sp. remains unaffected. Such a difference is likely to be associated with ecological, physiological and/or immunological factors influencing the ligulosed fish host.
Ecological factors are mainly associated with the frequency of contact between free-living cercarial stages and the fish target host. Only when the two occupy the same ‘space’ are infections more likely to take place (Combes et al., Reference Combes, Fournier, Moné and Theron1994). Therefore any effect that L. intestinalis may have on the fish that increases the amount of contact time with cercariae may promote changes in eyefluke occurrence. Ligulosed fish are known to have altered behaviour patterns, with infected fish tending to congregate closer to inshore areas (0–10 m) during July to December (Loot et al., Reference Loot, Brosse, Lek and Guégan2001), where molluscan intermediate hosts of eyeflukes commonly inhabit the increased masses of vegetation found on the bank margins. However, eyefluke infections of roach from White Swan Lake remain modest compared with other freshwater habitats, where prevalence levels of 95–100% have been recorded (Chappell et al., Reference Chandler1994). The present site is a managed habitat where most of the bankside vegetation is regularly cut back to improve angling activities. Only in the north end of the lake are more extensive reed beds allowed to flourish, and here a higher biodiversity of invertebrates, particularly aquatic insects, occurs (Chandler, Reference Chandler1994). It is possible that this unmanaged area of the lake may have attracted ligulosed roach as well as definitive bird and molluscan intermediate hosts of Diplostomum sp., facilitating transmission opportunities. In contrast, the occurrence of Tylodelphus sp. in ligulosed roach remained unchanged, which may indicate that bird and molluscan hosts for this species occur in other locations on the lake. Bouillon & Curtis (Reference Bouillon and Curtis1987) suggested that the risk of acquiring eyefluke infections is spatially related to the area traversed by the fish during its life.
Physiological effects can influence the ability of cercariae to penetrate, migrate and establish in the eyes of fish hosts. Compounds such as glycoproteins, present in mucus-covered fish, are necessary to initiate cercarial penetration (Haas, Reference Haas2003), while successful migration through the host body is dependent on various host-derived chemical cues for orientation and establishment in the eye (Haas, Reference Haas2003; Haas et al., Reference Haas, Wulff, Grabe, Meyer and Haeberlein2007). The migrating larvae of trematodes are known to adopt species-specific orientation strategies responding to diverse kinds of host signals and different concentration gradients of the same compounds, while following similar migration routes through the host (Haas et al., Reference Haas, Wulff, Grabe, Meyer and Haeberlein2007). It is possible that systemic pathological effects of L. intestinalis on the fish host may alter the composition and concentration of certain host compounds that are necessary for successful establishment of parasites in the eyes. Consequently, migrating larvae of Diplostomum sp. and Tylodelphus sp. are likely to have different responses to the same patho-physiological changes in ligulosed roach.
Changes to the immunological status of ligulosed fish may also be influential, where an intense cellular response to the plerocercoid, involving a number of specific and non-specific humeral components, is invoked (Hoole et al., Reference Hoole, Carter and Dufour2010). Similarly, eyeflukes, particularly Diplostomum spathaceum, have also been shown to induce an immune response in fish, although the parasite remains vulnerable only during its migration through the host body, as the eye is an immunological privileged site, thereby protecting it from any further defensive responses by the fish (Chappell, Reference Chappell1995). Changes in the prevalence of Diplostomum sp. in ligulosed roach may therefore be the result of immune modulation or reduced cellular activity caused by this co-infection, as recorded previously in some mammalian–helminth systems (Corrêa-Oliveira et al., Reference Corrêa-Oliveira, Golgher, Guilherme, Carvalho, Massara, Caldas, Colley and Gazzinelli2002).
In the present study, bilateral asymmetry was recorded in one of the eyefluke species, Tylodelphus sp., but only in non-ligulosed roach. Deviation from symmetry has been reported previously in eyeflukes from fish, although its occurrence lacks any consistency between studies (Johnson et al., Reference Johnson, Koprivnikar, Orlofske, Melbourne and Lafonte2014; Wayland & Chubb, Reference Wayland and Chubb2016). Mechanisms responsible are little understood but may include the effects of host morphology, physiology or mortality, alongside parasite mortality and responses to host-derived chemical cues during the migration of larval stages through the body (Johnson et al., Reference Johnson, Koprivnikar, Orlofske, Melbourne and Lafonte2014). Ligula intestinalis plerocercoid interference with the development of bilateral asymmetry of Tylodelphus sp. is likely due to one or more of these mechanisms being altered directly by this larval cestode or the patho-physiological changes it imposes on the host, and may, as discussed above, also be associated with changes in the prevalence of Diplostomum sp. in this roach population.
In conclusion, it seems likely that alterations in the incidence of eyeflukes are the result of ecological, physiological and immunological influences that L. intestinalis has on the host. The present study, undertaken under natural conditions, broadly supports the experimental results of Benesh & Kalbe (Reference Benesh and Kalbe2016) in a similar cestode–fish system, i.e. S. solidus–stickleback, and indicates that larval cestodes residing in the peritoneal cavity of fish can indirectly interact with other helminth species in the same host. Therefore, as ligulosis can achieve high levels of infection in fish (Sweeting, Reference Sweeting1977; Kennedy et al., Reference Kennedy, Shears and Shears2001; Zhokhov & Pugacheva, Reference Zhokhov and Pugacheva2012), the potential effects of co-occurring helminths on the ecology of parasites in wild fish populations should not be overlooked.
Financial support
This research received no specific grant from any funding agency, commercial or not-for-profit sectors.
Conflict of interest
None