


INTRODUCTION
Sensitivity analysis is an important part of mathematically modelling the system of biochemical reactions that constitute the cells, organs or whole body of a growing or lactating animal. In sensitivity analysis, as described by Baldwin (Reference Baldwin1996), the responses of key output variables of the model to changes in values of individual parameters, such as Vmax and Km in the biochemical equations, are quantified. The results may be presented graphically as model output v. parameter value. Sensitivity is defined as the slope of the response, where a higher slope indicates a greater sensitivity of the model to the value of that particular parameter. France & Thornley (Reference France and Thornley1984) suggest the calculation of an instantaneous slope from a 5% change (although the equation applies to other degrees of change) in the parameter value as:
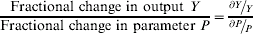
Sensitivity analysis, in addition to being conducted in silico on a mathematical model of a system, can also be conducted experimentally on the biological system itself. In this context, sensitivity analysis has been called metabolic control analysis (MCA). Imagine a series of consecutive biochemical reactions that result in formation of a product. The effect on flux through the pathway (i.e. product formation) of changing the Vmax or Km by administering specific inhibitors, activators, or overexpressing or silencing genes could be monitored. The fractional change in flux relative to fractional change in each enzyme's activity quantifies the degree of control each enzyme exerts over total pathway flux. The higher the control coefficient, the greater the impact of that enzyme in controlling pathway flux.
Fluxes through metabolic pathways are useful to measure, because it is considered, according to a reductionist analytical philosophy, that such fluxes explain or account for the aspect of whole-animal function that is of interest, such as daily milk yield, chemical composition of the milk, or growth rate. Beyond just measuring fluxes, identifying where the control over flux lies allows the system to be perturbed or, more precisely, engineered to bring about a desired change in the rate of milk production, composition of the milk, or growth rate. The common descriptor of biochemical control with which many are familiar is the designation of an enzymatic step as being rate-limiting to the pathway. MCA, however, is based upon the hypothesis that at any point in time the control over the rate of product formation is distributed (not necessarily equally) among all the components of the pathway. In other words, there are degrees of rate-limitation. The rate-limiting description bears the connotation that all of the control over the pathway flux is borne by this one step, which is a drastic oversimplification of how biochemical regulation operates. In fact, where there is regulation of an enzyme, say feedback inhibition of the first step in a pathway from a downstream metabolite, the flux control coefficient for product formation may actually be quite low (Kacser & Burns Reference Kacser and Burns1973). Increasing the amount of an enzyme that is regulated allosterically by feedback inhibition would be expected to have little effect on the rate of product formation. Thus, MCA introduces rigour into the language by which biochemical control is described and does not allow for the oversimplification implied by the term rate-limiting, which due to its rarity of occurrence, should be dropped from the lexicon.
Analysis of control points takes on a larger significance in the age of molecular biology where it is relatively commonplace to change the level of expression of a particular gene with the expectation that the flux through the pathway in which the gene product participates will change accordingly. Niederberger et al. (Reference Niederberger, Prasad, Miozzari and Kacser1992) examined the synthesis of tryptophan in yeast following over-expression of five enzymes of the synthetic pathway. Singly, expression of each enzyme was increased from 10 to 51 times the basal level, but the rate of tryptophan synthesis only increased to a maximum of 1·3 times wild-type. When all enzyme levels were increased simultaneously by 19- to 26-fold, tryptophan synthesis was increased by a factor of 9. The results indicate that control is distributed over many enzymes of the tryptophan synthesis pathway and that modification of tryptophan flux will not be successful if only one enzyme of the pathway is targeted for genetic manipulation.
The MCA perspective helps to explain apparent anomalies such as insulin-stimulated glucose disposal in mice in which the insulin-sensitive glucose transporter GLUT4 has been knocked out (Fueger et al. Reference Fueger, Li, Ayala, Shearer, Bracy, Charron, Rottman and Wasserman2007). The phenomenon does not require proposition of novel insulin-sensitive glucose transporters. Rather, GLUT4 exerts less than 100% of the control over insulin-stimulated glucose disposal, and an increase in intracellular glycogen synthesis and glycolytic flux under the influence of insulin would be expected to increase glucose uptake into tissues by any one of the insulin-insensitive transporters that facilitate glucose diffusion in both directions across the plasma membrane.
The distribution of flux control is apparent from recent genomic and proteomic studies where broad arrays of gene transcripts or proteins are quantified in tissue samples. Typically, many enzymes of a particular metabolic pathway or process are affected similarly by the experimentally imposed treatment. For example, O2 depletion of cells increased activities of all 11 glycolytic enzymes in macrophages and skeletal muscle cells (Robin et al. Reference Robin, Murphy and Theodore1984). During CLA-induced milk fat depression, all seven lipogenic enzymes evaluated were down-regulated in mammary expression (Baumgard et al. Reference Baumgard, Matitashvilli, Corl, Dwyer and Bauman2002). This redundancy is exploited in computer-assisted pathway analysis to identify, out of possibly hundreds of differentially expressed genes, which biochemical pathways appear to have been up- or down-regulated (Salomonis et al. Reference Salomonis, Hanspers, Zambon, Vranizan, Lawlor, Dahlquist, Doniger, Stuart, Conklin and Pico2007).
In dairy research, considerable effort is expended to manipulate the production, or efficiency of production, of the nutritive and bioactive components of milk. There are reports of cows producing ‘designer’ milk that is enriched in some of the many components naturally present in the medium (Boland et al. Reference Boland, MacGibbon and Hill2001; Playne et al. Reference Playne, Bennett and Smithers2003; Ward & German Reference Ward and German2004). This effort has benefited from the technologies of molecular biology and knowledge has increased exponentially about the discrete biochemical steps involved in milk synthesis. However, in order to engineer a desired change in milk composition, those parts of the milk synthetic pathways to change must be known. That knowledge is gained by identifying the proportion of metabolic control exerted by each step in the pathway. To date, two experiments have applied MCA to different aspects of milk synthesis (Xiao & Cant Reference Xiao and Cant2005; Wright et al. Reference Wright, Cant, Brenna and McBride2006). The objective of the present paper is to provide a brief overview of some of the tenets of MCA and review an example of its application in lactation biology, using as reference an examination of de novo fatty acid synthesis in bovine mammary homogenates (Wright et al. Reference Wright, Cant, Brenna and McBride2006).
METABOLIC CONTROL ANALYSIS: AN OVERVIEW
The development of MCA dates from the early 1970s. It was presented in comprehensive forms by Kacser & Burns (Reference Kacser and Burns1973) and Heinrich & Rapoport (Reference Heinrich and Rapoport1974). The readable account for non-mathematicians by Quant (Reference Quant1993) provides a good basis for using MCA, and experimental approaches to the technique have been given by Harper & Brand (Reference Harper and Brand1995).
The core elements of MCA, which are the basis for understanding the use of this approach experimentally, have been described by Fell (Reference Fell1992), and only the most salient are described herein. The first element of MCA is the flux control coefficient, which is a sensitivity coefficient defined, according to Eqn (1), as the fractional change in steady-state flux through the entire metabolic pathway (J) for an infinitesimal change in the activity of enzyme i (E i):

For a simple linear pathway, such as
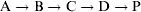
in which there is no allosteric or hormonal regulation of enzyme activity, the intuitive expectation might be that a 1% increase in activity (e.g. Vmax) of the first enzyme catalyzing the A→B reaction will result in a 1% increase in steady-state flux through the entire pathway producing P. However, the reversibility of enzymatic reactions counteracts this expectation. The effect of product accumulation on net flux through an enzymatic step is seldom taken into account in experimental measurements and in models thereof. However, all enzyme reactions are reversible and in entire systems, like a simple linear chain of enzymatic reactions, the intermediate metabolites can accumulate and, by mass action, stimulate the reverse flux. Thus, when the A→B flux is accelerated by 1%, B accumulates and stimulates both the B→C and B→A reactions. Due to the loss of B back to A, the increase in B→C will not be as large as 1%. And the stimulation will progressively diminish with each subsequent step, according to the specific kinetics by which substrate and product concentrations influence the velocities of forward and reverse reactions, respectively. In the end, the new steady-state rate of production of P may be considerably slower than the initial 1% increase in Vmax of E A, resulting in a control coefficient less than 1·0. What MCA of a real system provides, that sensitivity analysis of a simulation model generally does not, is these effects of enzyme reversibility and other unforeseen interactions between metabolite concentrations and enzyme activities. In fact, the results of MCA experiments could be used as test data to evaluate adequacy of simulation models.
In order to calculate control coefficients, the challenge experimentally is to measure the change in pathway flux and the change in enzyme activity as two separate processes. Very often flux is taken as a measure of enzyme activity, but the two are not synonymous, as shown above. Generally, the effects of enzyme perturbation on flux are measured on the whole system under study and the effects on enzyme activity are measured on the isolated enzyme, or calculated from the enzyme kinetic theory, for conditions equal to those in the whole system. The examples given in the current paper illustrate different approaches to solving the problem experimentally.
Flux control coefficients are described as system properties because the flux control coefficient of an enzyme can change when there are alterations in other parts of the pathway. For example, a hormone that influences the expression and phosphorylation state of a select number of enzymes will create a new basal state of intermediate concentrations from which the perturbations in E i will be evaluated and, consequently, yield different control coefficients.
The second fundamental element of MCA is the summation theorem that specifies that the sum of all the flux control coefficients in a linear pathway of n steps will equal 1:

In simple cases, the flux control coefficients lie between 0 and 1. A flux control coefficient value of 0 indicates that the enzyme has no control over the flux through the pathway, while a flux control coefficient value of 1 represents total control, the otherwise misleading rate-limiting enzyme. In branched metabolic pathways, it is possible for control coefficients to have values outside of this range (Fell Reference Fell1997). A negative flux control coefficient would occur if, for example, activity in one branch of the pathway had the effect of lowering the flux through the other branch of the pathway.
Kashiwaya et al. (Reference Kashiwaya, Sato, Tsuchiya, Thomas, Fell, Veech and Passonneau1994) examined the control of free glucose conversion to glycogen and lactate in perfused rat heart using MCA. They measured the metabolic fluxes, concentrations of all intermediates in the two branches of the pathway, forward Vmaxs and Kms for all 17 enzymes, and reverse Vmaxs and Kms for nine of those enzymes. From the data, and according to the Michaelis–Menten equations and displacements of the product/substrate ratios from the equilibria, the instantaneous slopes of each enzyme's velocity response to a change in its substrate concentration were predicted. These enzyme elasticities ( ) were converted to flux control coefficients by solving a set of simultaneous equations including the summation theorem (Eqn (4)) and a connectivity theorem that states that the sum of the control-elasticity products equals zero:

The elasticity approach based on enzyme kinetics is one alternative, not based on directly perturbing enzyme activities with activators, inhibitors or genetic modification, to separate the changes in pathway flux from changes in enzyme activity and obtain flux control coefficients. For glycogen synthesis in cardiac muscle, Kashiwaya et al. (Reference Kashiwaya, Sato, Tsuchiya, Thomas, Fell, Veech and Passonneau1994) estimated that glucose transport exerted 0·40 of the control and hexokinase exerted 0·59; phosphoglucoisomerase and glycogen phosphorylase exerted very little. Addition of insulin to the perfusate, which increases the Vmax of glucose transport, effected a reduction in the control coefficient for transport to less than 0·01.
When the steps of glucose transport and phosphorylation, glycogen synthesis, and glycolysis were lumped into three aggregate blocks of glucose metabolism, the control coefficients for the three blocks were estimated to be 0·58, 0·17 and 0·26, respectively (Kashiwaya et al. Reference Kashiwaya, Sato, Tsuchiya, Thomas, Fell, Veech and Passonneau1994). Because glycolysis only accounted for a quarter of the control over glucose disposal, those authors concluded that phosphofructokinase was not the rate-limiter many have supposed from the elaborate mechanisms that act to regulate its activity. Others have found similarly low coefficients of control over glucose disposal or glycolytic flux for phosphofructokinase (Meléndez-Hevia et al. Reference Meléndez-Hevia, Mateo and Torres1992; Jucker et al. Reference Jucker, Barucci and Shulman1999). The low coefficient does not indicate that the regulatory mechanisms, such as sigmoidal kinetics relative to its substrate fructose-6-phosphate, inhibition by citrate and ATP, activation by fructose-2,6-bisphosphate, etc. (Kemp & Markus Reference Kemp, Markus and Pilkis1990), are unimportant. Rather, the low control coefficient suggests that the glycolytic flux cannot be manipulated effectively by modifying the phosphofructokinase expression. Indeed, overexpression of phosphofructokinase in yeast and potatoes has had little effect on the rate of glycolysis (Davies & Brindle Reference Davies and Brindle1992; Thomas et al. Reference Thomas, Mooney, Burrell and Fell1997).
Transmembrane transport of glucose into cells has often been named the rate-limiting step in glucose metabolism (Kahn Reference Kahn1992; Ren et al. Reference Ren, Marshall, Gulve, Gao, Johnson, Holloszy and Mueckler1993). This hypothesis is of interest to lactation biologists because lactose is synthesized from glucose and lactose is the primary osmoregulator of milk, making it the primary determinant of milk volume. Wilde & Kuhn (Reference Wilde and Kuhn1981) found that glucose concentration inside mammary epithelial cells of rats was approximately three times lower than the Km for lactose synthesis and interpreted the difference to mean that glucose transport from the extracellular space was rate-limiting to lactose synthesis. Subsequently, Threadgold et al. (Reference Threadgold, Coore and Kuhn1982) found that rates of glucose transport and total glucose consumption by mammary acini in vitro were similar to each other. It was again concluded that transport is rate-limiting to glucose utilization. Neither conclusion was based on a direct test of the role of glucose transport in lactose synthesis by, for example, inhibiting or activating glucose transport. When phloretin was included at 100 μM in the incubation medium to inhibit facilitated glucose transport, glucose uptake fell by 61% of the control rate and lactose synthesis by 83% (Wilde & Kuhn Reference Wilde and Kuhn1981). This large response in lactose synthesis supports a role for glucose transport in control of flux to lactose. However, activation and inhibition of glucose transport and glycogen synthesis in muscle have indicated that transport of glucose is only partly responsible for the control of glucose utilization (Kashiwaya et al. Reference Kashiwaya, Sato, Tsuchiya, Thomas, Fell, Veech and Passonneau1994; Fisher et al. Reference Fisher, Nolte, Kawanaka, Han, Jones and Holloszy2002; Whitesell et al. Reference Whitesell, Ardehali, Printz, Beechem, Knobel, Piston, Granner, Van Der Meer, Perriott and May2003).
To evaluate the relationship between glucose transport and metabolism in bovine mammary epithelial cells, the Michaelis–Menten parameters of the three processes of glucose transport, glucose oxidation and lactose synthesis simultaneously in the same primary cell cultures (Xiao & Cant Reference Xiao and Cant2005) were estimated. Simulation of MCA, by effecting infinitesimal (0·3%) changes in the Vmax of transport, phosphorylation, isomerization, oxidation and lactose synthesis, revealed that transmembrane transport accounted for about 0·20 of the control of lactose synthesis, while phosphorylation accounted for approximately 0·80 of the control (Xiao & Cant Reference Xiao and Cant2005). It was concluded that future strategies to engineer desired levels of daily milk production should concentrate on manipulations of hexokinase activity that reflects the importance of phosphorylation, rather than the previous emphasis on transmembrane transport of glucose.
MCA IN BOVINE MAMMARY FATTY ACID SYNTHESIS EXPERIMENTS
One of the largest nutritional manipulations of milk composition in dairy cattle is the milk fat depression due to trans-fatty acid production in the rumen. Milk fat content may fall by more than 20 g/litre and the mRNA abundances of acetyl CoA carboxylase-α (ACC), fatty acid synthase (FAS), stearoyl-CoA desaturase, lipoprotein lipase, fatty acid binding protein, fatty acyl CoA ligase, glycerol phosphate acyl transferase and acylglycerol phosphate acyl transferase in mammary tissue fall similarly (Peterson et al. Reference Peterson, Matitashvili and Bauman2003). These enzymes are involved in de novo synthesis of fatty acids from acetate and butyrate, or transfer of long-chain fatty acids from blood to milk triacylglycerol.
Acetyl-CoA carboxylase-α has long been described as the rate-limiting enzyme for de novo fatty acid synthesis in mammary epithelial cells (Grummer Reference Grummer1991; Molenaar et al. Reference Molenaar, Mao, Oden and Seyfert2003). This characterization is based upon the regulatory properties of the enzyme. Short-term regulation is through an activating, polymerization effect of citrate, a depolymerizing effect of long-chain fatty acids, and reversible covalent phosphorylation by cyclic AMP-dependent protein kinase and AMP-activated protein kinase, which both inhibit, and an insulin-responsive kinase, which activates (Brownsey et al. Reference Brownsey, Boone, Elliott, Kulpa and Lee2006). Longer term regulation of the ACC-α activity is exerted at the levels of transcription and mRNA stability (Munday Reference Munday2002; Barber et al. Reference Barber, Price and Travers2005). Four promoters have been identified in mammalian ACC-α genes (Barber et al. Reference Barber, Price and Travers2005). Depending on the tissue and species of mammal, ACC-α is transcribed from different promoters, resulting in slightly different isoforms of the enzyme that share common catalytic and regulatory features. Promoter II is responsible for up-regulation of mammary ACC-α expression at the onset of lactation in rodents, whereas promoters IA and III are responsible in ruminants (Molenaar et al. Reference Molenaar, Mao, Oden and Seyfert2003; Barber et al. Reference Barber, Price and Travers2005). These promoters contain response elements to a carbohydrate-responsive factor and sterol responsive element binding protein-1.
Fatty acid synthase activity, on the other hand, is regulated almost exclusively at the transcriptional level (Sul & Wang Reference Sul and Wang1998) from signals induced by carbohydrate and fatty acid status. It is not subject to post-translational modification or allosteric regulation (Sul & Wang Reference Sul and Wang1998).
The flux control coefficient for ACC over lipogenesis in maize and barley was 0·54 (Page et al. Reference Page, Okada and Harwood1994). Fifty-fold overexpression of ACC in Escherichia coli resulted in a six-fold stimulation of fatty acid synthesis (Davis et al. Reference Davis, Solbiati and Cronan2000). Both of these observations attest to the importance of ACC in the control of fatty acid synthesis. However, neither its isolated regulatory properties, nor its high flux control coefficient in other organisms supports the hypothesis that ACC is the rate-limiting enzyme in de novo mammary fatty acid synthesis.
To test the hypothesis that ACC is rate-limiting, MCA was applied to the cytosolic steps of the lipogenic pathway (Wright et al. Reference Wright, Cant, Brenna and McBride2006) that are mediated by ACC-α and FAS:
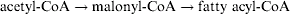
Activity of ACC in post-mitochondrial supernatants of homogenized mammary tissue was manipulated by titrating the effect of 0–10 μM avidin, a slowly irreversible inhibitor of biotin-dependent carboxylases (Duggleby et al. Reference Duggleby, Attwood, Wallace and Keech1982), on rates of fatty acid synthesis measured as incorporation of 1-14C acetate into ether-soluble lipid. Acetyl-CoA carboxylase activity was assayed in separate incubations as incorporation of H14CO3 into acid-stable products. Instantaneous slopes at 0 μM avidin were obtained for the changes with avidin concentration in both flux and enzyme activity, as proportions of their respective uninhibited values. The ratio of these initial slopes yielded a flux control coefficient of 0·63 for ACC (Wright et al. Reference Wright, Cant, Brenna and McBride2006). By the summation theorem (Eqn (4)), the control coefficient for FAS was 0·37. The conclusion is that ACC exerts the majority of control over fatty acid synthesis by the mammary ACC–FAS sequence but it is not rate-limiting; FAS also exerts control over the flux. An increase in FAS activity, independent of a change in ACC, would be expected to influence the rate of fat synthesis.
The cytosolic ACC–FAS sequence is a truncated portion of the complete mammary pathway of de novo lipogenesis that also includes glycolytic enzymes and glycerol phosphate dehydrogenase to form α-glycerol phosphate, and microsomal acyltransferases to synthesize triacylglycerols. The external supply of NADPH for FAS could also influence the level of control this enzyme exerts. And once triacylglycerols are synthesized, they are secreted apically by an apocrine mechanism that is still poorly understood but involves a host of enzyme and protein interactions (Heid & Keenan Reference Heid and Keenan2005). Thus, identification of all metabolic steps to which milk fat production is sensitive could extend well beyond the core pathway from acetate to long-chain fatty acids. Future progress in the techniques of metabolomics to identify concentrations of all intermediate metabolites in a pathway, and proteomics to quantify concentrations of all enzymes, will facilitate the calculation of control coefficients by the elasticity approach (Eqn (5)) for more complex pathways than have hitherto been subjected to the analysis. The results of MCA in mammary homogenates should be augmented by such investigations in whole-cell preparations. The values of the flux control coefficients for ACC and FAS are probably reduced in MCA experiments that include a broader array of potential control points present in a more complete lipogenic pathway.
CONClUSIONS
MCA is a useful tool for biologists to identify steps of metabolic pathways that exert significant control over flux, defined as those to which the flux is sensitive. These steps are not necessarily those for which multiple mechanisms of short- and long-term regulation have been defined, such as the phosphofructokinase reaction. Rather, they are points whose perturbation is most likely to result in a change in output of product. Application of MCA to mammary metabolism in laboratories has provided evidence that mammary hexokinase activity exerts more control than trans-membrane entry of glucose over lactose synthesis (Xiao & Cant Reference Xiao and Cant2005), and that ACC is not the only enzyme controlling de novo fatty acid synthesis (Wright et al. Reference Wright, Cant, Brenna and McBride2006). In future, MCA could be used to integrate pathway flux data with large-scale metabolite and protein concentration measurements to advance the possibility for metabolic engineering of designer milk from dairy animals.


