




Nutrition is an evolving science in which combinations of observational and mechanistic data are interpreted in the context of relationships between food intake and health outcomes(Reference Mozaffarian, Rosenberg and Uauy1). The high level of complexity and heterogeneity in not only foods but also within and between individuals have always been limiting factors in drawing general conclusions on what constitutes ‘healthy’ or ‘unhealthy’ foods. Consequently, the shaping of public health messages requires a trade-off between scientific robustness and communication clarity. Over the past decades, two different approaches have been pursued in parallel. One emphasises food groups such as grains, fruits and vegetables, dairy, etc. and advocates for an appropriate balance within the total diet. This is accompanied by recommendations for the number of daily serves of specific food groups and is typically illustrated by food plates or pyramids as communication aids(Reference Herforth, Arimond and Alvarez-Sanchez2,Reference Rong, Liao and Zhou3) . The second approach is based on the molecular composition and (calculated) energy content of foods, with particular emphasis on contents of carbohydrates, proteins, fats and fibre. Nutrition information panels and recommended daily intakes of specific nutrient types are examples of outcomes from this approach(Reference Afroza, Abrar and Nowar4,Reference Salesse, Eldridge and Mak5) . However, an emphasis on individual nutrients is often difficult to reconcile with the more general nutrition messaging around a balance of whole foods as the core of a healthy diet.
While molecular composition is one aspect of the nutritional value of foods, on its own it does not capture the benefits of a diet based on whole foods. There are three major causes for this. One is the over-simplification that all types of proteins, fats or carbohydrates have equivalent energy contents. A second is the multitude of minor ‘bioactive’ components in whole (minimally processed) foods that are not captured by current composition analyses but are likely to contribute to health benefits. The third is that a molecular description fails to take account of the macroscopic food structure (matrix) and how this controls the release of nutrients after ingestion(Reference Grundy, Edwards and Mackie6–Reference Gidley8). One aspect of this last deficiency is the assignment of energy to carbohydrates, lipids and proteins in foods based on the assumption that all macronutrients are fully digested by the end of the small intestine. However, one of the features of many whole (minimally processed) foods is that plant (or animal) tissue structures may limit digestion by the end of the small intestine and allow some macronutrients to become available for fermentation in the large intestine with a reduction in energy available to the host or, if not fermented, excreted with no energy to the host. This is a long-recognised problem for some foods(Reference Capuano, Oliviero and Fogliano9) such as whole nuts where the robust tissue structure protects some of the high lipid content from digestion and to a lesser extent fermentation. This leads to an overestimation of available energy content based on macronutrient content alone(Reference Nikodijevic, Probst and Tan10,Reference Novotny, Gebauer and Baer11) .
The disconnect between nutrient and whole food nutrition messaging approaches has created a vacuum which has been filled by alternative or additional narratives, such as adherence to a particular diet type (some with good scientific support, others more passing fads) and recently the emergence of ultraprocessing as a classification proposed to be an arbiter of ‘healthy’ vs ‘unhealthy’ food(Reference Monteiro, Louzada and Steele-Martinez12). As many have pointed out, defining nutritional value based on whether a food was prepared in a factory or elsewhere does not stand up to detailed scrutiny(Reference Lockyer, Forde and Adams13–Reference Forde15). Nevertheless, the correlations between ultraprocessed food intake and (biomarkers for) health risks may be strong, reflecting the continuing change of the place of foods in society from something that is enjoyed over extended mealtimes towards refuelling by time-poor consumers. A common feature of processed (‘ultra’ or otherwise) foods is that both digesta passage rate and nutrient release and absorption rates are typically increased compared with equivalent less processed foods. This combination of passage rate and nutrient release/absorption rates is captured by the term digesta dynamics.
One aim of this narrative review is to examine whether a combination of molecular composition and digesta dynamics can explain the observed correlations between diets rich in whole (minimally processed) foods and reduced risks of non-communicable chronic conditions. A second aim is to examine the idea that the term ‘ultraprocessed food’ is a useful branding tool for general nutrition messaging but less appropriate for classifying the nutritional value of individual foods.
Digesta dynamics
The journey of ingested food through the digestive tract involves four discrete stages, namely oral, gastric, small intestinal and large intestinal processing. Each of these stages has characteristic effects on (i) residual food structure, (ii) digestion/fermentation and absorption of nutrients and (iii) timescales of passage. Digesta dynamics is used here as a term to capture the interplay between passage timescales and the release/absorption of nutrients as mediated by food structure and composition. The biochemical and biophysical processes that occur in each of the digestive tract sections are well understood, but nutrition science does not often consider these processes in terms of the timescales that they occur over or the influences of previous stages of gastrointestinal processing. A greater appreciation of the temporal consequences of digestion for different foods can go a long way to explaining the nutritional impacts of eating whole foods and of processing whether in the kitchen or the factory.
The major non-communicable chronic conditions(Reference Chew, Ng and Tan16) that nutrition can play a role in reducing the risks of are intimately linked to digesta dynamics. The best-known example is probably the relationship between post-prandial glucose excursions and insulin responses as a risk factor for type 2 diabetes. Unsurprisingly, diet quality is the top predictor of type 2 diabetes risk globally(Reference O’Hearn, Lara-Castor and Cudhea17). The timescale over which glucose is absorbed in the small intestine is dependent on a combination of (i) any delay caused by gastric transit, (ii) release of sugars from food matrices in the small intestine and (iii) the digestion of starches by salivary and pancreatic amylases. Each of these factors is influenced by the architecture of (solid) foods and its extent of modification by oral and gastric processing.
A second example that is garnering strong public interest is the control of satiation and satiety(Reference Ni, Smyth and Cozzolino18) as an approach to weight management and reduction of risks for type 2 diabetes and other non-communicable diseases. In this case, food architecture has effects on both eating rate and gastric transit times and therefore the rate at which digesta is passed to the small intestine as one mechanism for prolonging the timescale of nutrient absorption and reducing the drive to continue eating (satiation) and to start eating again (satiety). Retention of digesta in the stomach can also be influenced by hormone signals from the distal small intestine triggered by nutrient absorption at the ileum, in effect alerting the stomach to the fact that active digestion is still occurring so there is less need for more digesta to be passed to the small intestine. Such signals not only influence gastric processing but also neurological processes related to satiety perception. Agonists for one such signalling hormone (glucagon-like peptide-1 (GLP-1)) are the basis for recently introduced drugs targeting diabetes and weight management. Whilst these drugs are proposed to function by binding to receptors in the brain(Reference Nauck, Quast and Wefers19), foods that have prolonged digesta dynamics generate transient signals via GLP-1 and other hormones that act as a natural short-term satiety regulation mechanism.
A third example is the partitioning of macronutrients in food/digesta between enzyme digestion and absorption in the small intestine and microbial fermentation (mostly) in the large intestine. Here digesta dynamics are critical, as the macronutrient content of residual digesta at the end of the small intestine is determined by the amount of enzymic digestion that occurs over a timescale determined by the passage rate from stomach exit to large intestine entry. Macronutrients that escape digestion in the small intestine are not only available to nourish the large intestinal microbiome but also reduce the amounts of e.g. glucose and fatty acids that are absorbed. This effect is a particularly important for foods containing intact plant cellular structures such as nuts, wholegrains and some legume foods.
Digesta dynamics also provides a framework for appreciating the evolutionary development of the human digestive tract. With a heritage as hunters and gatherers, there is a reasonable logic to identifying slow digestion over extended timeframes as an evolutionary advantage. Control points such as exit from the stomach, the combined action of enzymes and microbes to harness nutrients from relatively unprocessed food and hormonal mechanisms to control digesta passage and manage peaks and troughs in nutrient availability, can be envisaged to confer benefits to a species evolving in the context of its available but limited food resources.
In contrast to the whole (minimally processed) plant- and animal-based foods that our species evolved with, modern foods are often based on refined ingredients that are combined by processing. There are good historical reasons why this is so, primarily based on the greater storage stability of refined ingredients such as oils, sugars or flours compared with whole plant and animal foods. In previous centuries this was an important consideration for food security and led to first kitchen and then factory foods based on processing of ingredient combinations. From the perspective of digesta dynamics, the general issue with foods derived from combining refined ingredients compared with whole (minimally processed) plant or animal foods is that they tend to be disassembled more rapidly in the digestive tract. Processed foods therefore often have faster nutrient delivery less satiation and satiety(Reference Fardet20) and are rarely able to limit digestion sufficiently to make macronutrients available to the large intestinal microbiome. As noted in 2005, ‘The evolutionary collision of our ancient genome with the nutritional qualities of recently introduced foods may underlie many of the chronic diseases of Western civilisation’(Reference Cordain, Eaton and Sebastian21). With the economic development and associated nutrition transitions(Reference Bodirsky, Dietrich and Martinelli22) that have occurred across much of the world in the intervening two decades, this statement can now be generalised to many societies.
Over the past fifty years, globalised foods and fast-food restaurant chains offering instant availability have led to an increase in processed food intake across many parts of the world. This has been driven by time-poor consumers and reinforced by branding that seeks to achieve customer loyalty. In many cases the nutrient composition and assembled nature of these foods lead to low nutritional value, so it is reasonable to expect them to be subject to scrutiny. The most high-profile attempt to do so is the NOVA classification(Reference Monteiro, Louzada and Steele-Martinez12) that has been used to identify factory-made ‘ultraprocessed’ foods as particular culprits in increasing non-communicable disease (NCD) risks. The sustained and continuing increases in both NOVA-classified ultraprocessed food (UPF) intake and disease burdens can result in strong correlations(Reference Gonzalez-Gil, Matta and Morales Berstein23,Reference Juul, Martinez-Steele and Parekh24) , but the question remains whether there are direct cause-and-effect relationships(Reference Louie14,Reference Whelan, Bancil and Lindsay25,Reference Tobias and Hall26) .
Proposed mechanisms that may underpin the correlations between UPF consumption and NCD risk are generally of three types, namely high levels of undesirable nutrients (e.g. sugar, saturated fat, salt), weak food matrix structures and additives used in industrial food processing(Reference Juul, Martinez-Steele and Parekh24,Reference Scrinis and Monteiro27) . For the first of these (nutrient content) there is little doubt that this is a major factor, the second (matrix effects) impacts nutritional value by influencing digesta dynamics, but the evidence for the third (industrial additives) is weak at best. All industrially used food additives have been assessed to be safe to use by agencies such as the European Food Safety Authority or the US Food and Drug Administration, and there is no convincing evidence that these additives are directly involved in increasing NCD risk(Reference Whelan, Bancil and Lindsay25,Reference Besedin, Van and Besedin28) . Unfortunately, a main focus of NOVA protagonists is on the preservatives, colours, texturisers and other additives used in factory-processed foods, partly because this is the only point of differentiation from kitchen-processed analogues that are not defined as UPFs. In contrast, a combination of nutrient composition and digesta dynamics provides a coherent framework for understanding the food factors that contribute to NCD risk, with the consequence that the place of food processing (‘factory’ vs ‘kitchen’) may not be a critical factor from a mechanistic standpoint.
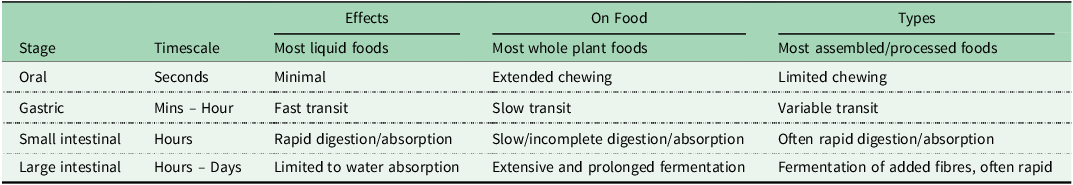
The following sections discuss digesta dynamics firstly from the perspective of each of oral, gastric, small intestinal and large intestinal processing (see Table 1 for a simplified summary), secondly as a concept with the potential to play a larger role in nutrition messaging and thirdly as a scientific framework to explain the effects of food processing on nutritional outcomes. This could provide a more mechanism-based alternative to the degree/place of processing as a categorisation and labelling tool.
Overview of timescales involved in sequential processing of food in the digestive tract and typical differences in response from liquid, plant-based and assembled/processed foods

Table 1. Long description
A table comparing the effects of different food types on digestion across various stages. The table has four rows and four columns. The columns are labeled Stage, Timescale, Effects, On Food, and Types. The rows are labeled Oral, Gastric, Small intestinal, and Large intestinal. The table details the timescale, effects on liquid foods, effects on whole plant foods, and types of processed foods for each stage of digestion. Row 1: Oral, Seconds, Minimal, Extended chewing, Limited chewing. Row 2: Gastric, Mins – Hour, Fast transit, Slow transit, Variable transit. Row 3: Small intestinal, Hours, Rapid digestion/absorption, Slow/incomplete digestion/absorption, Often rapid digestion/absorption. Row 4: Large intestinal, Hours – Days, Limited to water absorption, Extensive and prolonged fermentation, Fermentation of added fibres, often rapid.
Oral processing of food
Effects of oral processing on foods prior to swallowing can have marked effects on subsequent digestion properties for solid foods. The general features of oral processing for solid foods are size reduction by chewing and incorporation of saliva into a bolus that is then able to be swallowed safely(Reference Witt and Stokes29). The main biochemical consequence is the incorporation of salivary amylase into the food bolus that can initiate starch digestion in the mouth with continued action in the stomach(Reference Dhital, Warren and Butterworth30). The major matrix effects are the extent and ease of particle size reduction through mastication. Greater particle size reduction can lead to nutrients becoming more available for digestion/absorption, particularly for whole (minimally processed) foods where macronutrients are often cellularly encapsulated(Reference Mandalari, Parker and Grundy31,Reference Ranawana, Monro and Mishra32) . Foods with textures that lend themselves to easy mastication are associated with faster eating rates and can lead to greater consumption than analogous foods that are more difficult to masticate(Reference Forde15), as has recently been demonstrated in a clinical trial(Reference Forde, Heuven and van Bruinessen33). Compared with solid foods, liquid foods have short oral residence times and are typically swallowed with limited dilution or mixing. This makes liquid foods easier to consume than solid foods(Reference de Graaf34). A well-known example of this is the relative ease of drinking the juice (and pulp) from several fruits that it would not be possible to eat as intact fruit.
The effect of variations in oral processing outcomes both because of food texture and individual differences (‘coarse’ vs ‘fine’ chewers) leads to challenges in representing oral processing as the first step of in vitro digestion models(Reference Brodkorb, Egger and Alminger35). Routine lab methods such as grinding are inevitably limited in their ability to replicate the complexities and individual variation involved in mastication. Alternatives such as using ‘chew and spit’ methods may be more representative for an individual case but are clearly not suitable for routine assessment. One potential approach would be to use a range of e.g. three different in vitro oral processing conditions to represent the natural range found across populations.
Gastric digesta dynamics
Clear differences between liquid and solid food digesta are also expected in the stomach, with liquids able to readily pass through to the small intestine if they are not impeded by a high viscosity. Solids usually require further size breakdown and/or dilution as the size limit for pyloric sphincter passage to the small intestine is 1–2 mm, and chewing does not usually break solid foods to such small sizes. Viscosity is the other important physical parameter limiting exit from the stomach(Reference Liu, Jin and Wilde36), with foods that form viscous/structured material in the stomach being released slowly. Two well-known examples of this are wholegrains compared with refined grains(Reference Pletsch and Hamaker37) and the casein component of dairy foods which coagulates in the low pH conditions(Reference Zhang, Wilde and McClements38). In these and other cases of extended gastric transit time(Reference Ranawana, Clegg and Shafat39), nutrient delivery occurs over a longer time frame, and stretch receptors in the stomach can generate satiation signals to limit further intake. With the stomach acting like a digestion-preparing holding tank including acid- and pepsin-mediated digesta breakdown, it plays a key role in determining the temporal consequences of eating different food types with transit times ranging from minutes to hours. Whole (minimally processed) plant- and animal-based foods have many of the features associated with extended gastric transit times, whereas processed/assembled foods are often readily broken down to a form that can pass quickly to the small intestine.
Small intestinal processing and digesta dynamics
The primary processes that occur in the small intestine are the enzymic digestion of macronutrients and the absorption of nutrients, digestion products and water. Most enzyme activity is secreted into the first part of the small intestine as pancreatin containing proteases, lipases and alpha amylase along with bile salts for emulsification. Further digestive enzymes are associated with the intestinal epithelial cells (brush border). The rate of nutrient absorption (bioavailability(Reference Nicholas, Tone and Beal40)) depends on the bioaccessibility(Reference Grundy, Moughan and Wilde41) of nutrients from solid digesta and the rate of macronutrient enzyme digestion, with absorption of major nutrients only likely to be rate-determining for liquid foods. The small intestine has a very high surface area (often envisaged as being similar in size to a tennis court) and a transit time of hours that enables the efficient absorption of nutrients from the relatively unprocessed foods that our ancestors evolved with.
The often rapidly absorbed nutrients from liquid and assembled foods may only use the first part of the small intestine. Slower absorption due to restricted bioaccessibility and/or slow enzymic digestion will use more of the small intestine and smooth the uptake of e.g. glucose, amino acids and fatty acids so that the body is not overwhelmed leading to undesirable peaks and troughs. Nutrient absorption that is delayed until the end of the small intestine also triggers satiety hormones such as GLP-1 and others to signal that further food is not necessary.
The site of nutrient absorption depends on the interplay between nutrient-specific digestion/release rate and a passage rate driven by muscular peristalsis that can vary both between individuals and over time for an individual. One important consequence of this interplay is that, because there is no barrier controlling passage between small and large intestinal environments, any macronutrients that have not been digested enzymically and any absorbable nutrients that have not been released from digesta particles will pass into the large intestine. Whole (minimally processed) food structures(Reference Duijsens, Castillo and Verkempinck42), particularly plant cellular structures(Reference Dhital, Bhattarai and Gorham43,Reference Bhattarai, Dhital and Mense44) , are a prime example as intact plant cells are bounded by cell walls that are resistant to human digestive enzymes and can prevent or delay enzymes from accessing intracellular macronutrients and release of intracellular micronutrients. This can result in major differences in nutrient absorption rates and satiety hormone signalling for e.g. whole legume foods with intact plant cellular structures compared with puree/paste forms with broken cell walls but identical composition(Reference Cai, Tejpal and Tashkova45).
Large intestinal fermentation dynamics
In the large intestine, further digestive processing occurs, water and remaining nutrients are available for absorption and waste materials are excreted. The timescales over which these processes occur (typically hours to days) are influenced by prior processing of food through each of oral, gastric and small intestinal phases. The primary digestive processes in the large intestine are carried out by the resident microflora (microbiome) comprising many and diverse species containing a very wide range of potential digestive enzymes(Reference Fan and Pedersen46). Thus, many nutrients that were unable to be absorbed in the small intestine or macronutrients that remained undigested because of encapsulation effects are available as energy and metabolite sources for gut microbes. This is a mutually beneficial relationship, with major microbial metabolites such as the short-chain fatty acids (SCFA) acetate, propionate and butyrate being absorbed by the host. The complex dynamic between host and gut microbes is now recognised as playing a central role in human nutrition and health(Reference Dagbasi, Cai and Hirdaramani47) e.g. via gut-brain axis signalling.
The dynamics of large intestinal fermentation are a consequence of digesta composition and microbiome capability. Small soluble carbohydrates and related molecules are readily fermented and result in rapid production of gas and acid that can cause discomfort (gas) or more lasting damage (acid). For individuals that lack sufficient lactose-hydrolysing enzyme activities in the small intestine, this is manifested as lactose intolerance. More generally, FODMAPS (Fermentable Oligosaccharides, Disaccharides, Monosaccharides and Polyols) are recognised as being major sources of rapid fermentation. Slower fermentation is usually associated with plant cell wall material (often termed dietary fibre). For any macronutrients encapsulated in plant cellular foods, this fermentation also makes them available for fermentation. In general, more hydrated and swollen cell wall components such as pectins are typically fermented over a short timescale, with less hydrated and compact components such as cellulose fibre taking longer to ferment(Reference Yao, Flanagan and Williams48). Similar effects are seen for isolated solutions and gel particles of polysaccharides such as pectin and alginate, with gelation slowing the rate of in vitro fermentation(Reference Li, Shewan and Flanagan49).
Fermentation of carbohydrates is beneficial for a healthy gut as the SCFA produced prevents the pH from rising and thereby limits opportunistic pathogens. In addition, the SCFA butyrate is an important fuel for epithelial cells ensuring healthy functioning and reducing the risk of colon cancer. Whilst carbohydrates are considered the preferred source of nutritional energy, if supplies are exhausted, microbes can move to mucin from the gut lining or residual dietary protein as energy sources(Reference Davis, Bryant and Gibson50). However, depletion of mucin risks exposing underlying epithelial cells to infection or toxins, and fermentation of protein can result in harmful nitrogen-based, sulphur-based, phenolic and other metabolites.
Maintaining carbohydrate fermentation throughout the large intestine seems to be the ideal for both gut and systemic health and is a natural consequence of consuming a variety of plant foods with their diverse cell wall components and architectures(Reference Yao, Flanagan and Williams48,Reference Modasia, Spiller and Warren51) . Assembled foods struggle to achieve the same functionality even with added dietary fibre as this tends to be of a single type with a specific fermentation rate. Furthermore, added fibres are often selected for a lack of impact on food texture so tend to be of low molecular size (low viscosity) and therefore rapidly fermentable and not available to the distal large intestine. A further consideration is that colon cancers tend to be found towards the end of the large intestine consistent with a lack of slowly fermentable digesta as a risk factor.
The speed with which residual digesta is moved through the large intestine(Reference Roager, Hansen and Bahl52) is also related to the speed of fermentation of dietary fibres. Rapid fermentation is accompanied by associated water uptake and can lead to digesta that is too hard for passage and excretion i.e. constipation. Slower fermentation causes more water to be retained in digesta as fibre is generally highly hydrated. Not only does this ease passage but also stimulates the muscular movements needed for controlled excretion(Reference Roager, Hansen and Bahl52,Reference Cremer, Arnoldini and Hwa53) . Digesta dynamics in the large intestine may have been less studied than for oral, gastric or small intestinal phases but the extended timescale in the large intestine (usually tens of hours) means that there is more time to influence nutrition and health outcomes through the combination of (particularly) dietary fibre type with fermentation and water uptake rates.
Digesta dynamics in nutrition messaging
Two general benefits of integrating the concepts of digesta dynamics into nutrition messaging can be envisaged. One is to provide the link between the two current narratives based on either nutrient composition or food group/type. The second is to encourage consumers to be more aware of the processes that occur after eating food and the consequences of food choices on nutritional outcomes based on this enhanced understanding.
The current approaches to defining the nutritional value of foods and diets based on either molecular composition or food groups has led to a duality of messages that are often difficult to reconcile. Messaging based on composition highlights the benefits and drawbacks of specific nutrient types and was the dominant approach in the second half of the last century(Reference Mozaffarian, Rosenberg and Uauy1). This led to attempts at associating single (macro)nutrients with specific nutritional outcomes both positive and negative. For example, benefits of dietary fibre intake were identified based on compositional analysis of diets from populations with low levels of non-communicable diseases. A similar approach led to the proposal that dietary fat intake was a contributor to cardiovascular and other diseases, resulting in the popularisation of low-fat products that often replaced fat with structured carbohydrates. The next wave saw carbohydrates being identified as responsible for health risks and the move towards low-carb foods and diets.
Single macronutrient approaches are now recognised as being too simplistic, with more emphasis on the balance between macronutrients. This has led to categorisation of foods in terms of macronutrient balance, particularly protein and carbohydrate in e.g. a nutritional geometry approach(Reference Raubenheimer and Simpson54). Here, protein is proposed as the primary driver that animals including humans control their intake of (the protein leverage hypothesis(Reference Raubenheimer and Simpson55)) with negative human health implications if food choices lead to this protein being diluted with excess carbohydrate and/or fat. Whilst this approach has the benefit of being able to represent human and animal foods in two-dimensional plots, it does not take account of the clear effects of food processing on nutritional outcomes for the same macronutrient composition e.g. intact fruits vs juices; cellular nut/legume particles vs broken cells; whole grains vs flours.
A common feature of nutrient-based messaging is that accurate and reliable composition data can be determined by robust and established standard methods. This leads to a numerical/quantitative approach to nutrition messaging, as exemplified on food labels. Although this provides a sound foundation for regulators and communicators, it is currently insufficient to define the nutritional value of individual foods or their combination in diets, because it fails to take account of the effects of digesta dynamics.
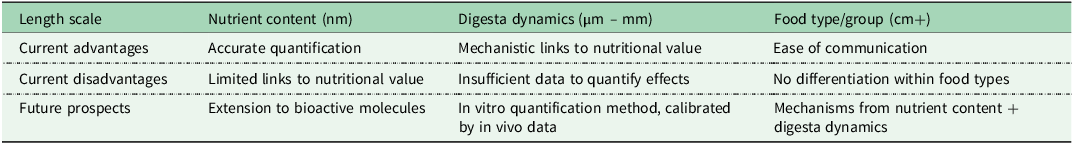
Nutrition messaging based on food groups/types is more qualitative as it is often difficult to quantify what a ‘serve’ is of a certain food type and many foods are composites of multiple food types or are ingredient-based and defy easy classification or quantification. Nevertheless, the strong correlations found in epidemiology studies between whole (minimally processed) food intake and reduced risks of NCDs provide a sound rationale for emphasising diets based on a balanced combination of whole foods. The qualitative (or at best semi-quantitative) nature of this strand of messaging lends itself more to images than to data as a medium of communication and has the benefit that consumers can readily identify with images of food types whereas molecular composition is a more abstract concept. A summary of the current approaches and potential introduction of digesta dynamics to nutrition messaging is shown in Table 2.
Overview of differences and relationships between current nutrition messaging approaches (nutrient content and food type/group including level of processing) and proposed additional messaging approach (digesta dynamics)

Table 2. Long description
A table with three rows and three columns comparing current advantages, disadvantages, and future prospects of nutrition messaging approaches across nutrient content, digesta dynamics, and food type/group scales. The columns are labeled Length scale, Nutrient content (nm), Digesta dynamics (µm – mm), and Food type/group (cm+). The rows are labeled Current advantages, Current disadvantages, and Future prospects. Current advantages include accurate quantification for nutrient content, mechanistic links to nutritional value for digesta dynamics, and ease of communication for food type/group. Current disadvantages include limited links to nutritional value for nutrient content, insufficient data to quantify effects for digesta dynamics, and no differentiation within food types for food type/group. Future prospects include extension to bioactive molecules for nutrient content, in vitro quantification method calibrated by in vivo data for digesta dynamics, and mechanisms from nutrient content + digesta dynamics for food type/group.
The general awareness levels of the food pyramid and particularly the meal plate communication tools coupled with the recognisable features of whole (minimally processed) foods is a type of branding mechanism in the sense that it provides an emotional connection to people in the way that fat, protein or carbohydrate content does not. A case can be made that a similar emotional connection has been established through the nomenclature of ultraprocessed food. The resonance of the term ‘ultraprocessed’ with consumers has established a brand position based on the unattractive sound of ‘ultra’ as a word applied to differentiate foods made in factories from those made in kitchens. A deeper emotional connection may also be caused by the accompanying narrative that ‘industry’ is responsible for producing foods with associated health risks. Identifying an outsider (‘industry’) as the cause of harm provides a common enemy that can be blamed for diet-related health risks. In this context, the ultraprocessed nomenclature is likely to have more cut-through than the identification of core (= ‘healthy’) and discretionary (= ‘unhealthy’) foods as discretion may be perceived as a personal choice whereas UPFs are ‘forced’ on consumers by ‘industry’. The language of UPFs is therefore a powerful communication tool even if lacks clarity of definition and struggles to articulate cause-and-effect mechanisms. There is little doubt that reducing the intake of industrially processed food in favour of whole (minimally processed) and kitchen-cooked food would enhance nutritional status. However, the lack of a credible mechanism distinguishing factory-processed from equivalent kitchen-processed foods means that UPF should be used as a qualitative or descriptive term rather than a quantitative or categorising term.
Digesta dynamics can be used to bridge the quantitative nutrient approach and the qualitative food type and processing approach to communication. The impact of food on nutritional and health status is based on the cumulative effects of all foods consumed and how the body manages absorbed nutrients. This involves both quantity and quality aspects as influenced by digesta dynamics. The quantity of food/nutrients consumed can be influenced strongly by (a) ease of chewing/swallowing, gastric transit time and consequent satiation acting as a limit to meal size and (b) timescales of digestion, absorption and fermentation influencing satiety and the subsequent onset of hunger. An example of the first influence that is straightforward to communicate is the difference in the amounts of fruits and vegetables that are easy to consume fresh (unprocessed) compared with juices made from the same components. The liquid form of juices leads to limited oral processing and is expected to result in short gastric transit times. In contrast, fresh (unprocessed) fruits and vegetables require significant oral processing and their particulate nature after swallowing is expected to result in extended gastric transit time limiting the desire for further ingestion. This example also lends itself to practical demonstrations of the effect of food architecture on digesta dynamics and satiation. For example, most people will struggle to eat two or three apples or oranges, but the juice from these apples or oranges (including the pulp) can usually be readily and rapidly consumed.
Impacts of digesta dynamics on absorption and fermentation take place over longer (hours to tens of hours) timescales, with small intestinal processing primarily influencing next meal (2–6 h) effects and fermentation effects likely to influence next day (12–24 h) effects that are more difficult to identify. The combination of gastric and small intestinal digesta dynamics has been shown to have marked effects on e.g. wheat- and chickpea-based foods depending on their particle size. Larger particles result in slower absorption of glucose from starch digestion and (for chickpea) increased secretion of GLP-1 and other ‘satiety’ hormones(Reference Cai, Tejpal and Tashkova45,Reference Edwards, Ryden and Mandalari56) .
More generally, nutrition communication that encourages a greater understanding of timescales involved in food digestion could become a platform for discussing why whole (minimally processed) foods have more nutritional value than many assembled foods. This could also cause consumers to think more about how long they spend eating and the likelihood that foods designed to be easy to eat are often easy to over-eat at least partly because of their rapid oral and gastric processing. Related to this, one of the proposed benefits of Mediterranean diets is the extended mealtimes that are traditional in that region. This allows satiation signals from gastric and initial small intestinal processing to be generated and acted upon during the meal rather than eating so rapidly that satiation signals are generated too late to influence intake.
Although digesta dynamics together with nutrient composition should be sufficient to explain the principles underlying NCD risk management through dietary choices, at this stage it is a largely qualitative and descriptive concept rather than a quantitative and predictive one. In this way, digesta dynamics should be seen currently as an adjunct to food plates/pyramids as an explanatory tool that illustrates the benefits of nutrient-balanced whole food combinations over assembled/processed foods with undesirable nutrient contents.
Digesta dynamics for food classification
While it is combinations of foods in a dietary context that determine overall nutritional status and corresponding NCD risk, the contribution of individual foods is important to consider, not least because this is often the unit that is purchased. Regulated or mandated classification of individual foods seeks to provide guidance to consumers and can be either quantitative or qualitative. Quantitative classifications include nutrition information panels, specific attributes such as Glycemic Index and star ratings or similar that quantify a basket of nutrition indicators to numerically classify individual foods. Qualitative or semi-quantitative classifications include traffic light signals, identification of foods as being e.g. ‘a source of’ or ‘a good source of’ positive nutrients such as protein or fibre and endorsements by e.g. heart associations or other health-related agencies.
Nutrition information panels currently list contents of major components, particularly macronutrients, typically on a gram per hundred gram and/or gram per serve basis. As discussed above, addition of information on digesta dynamics would serve to segregate nutritional outcomes beyond composition. In practice this is currently very difficult to do as there is limited quantitative in vivo data available on digesta dynamics at the food level. As suggested elsewhere(Reference Gidley57,Reference Gidley58) , the best current compromise would be to estimate nutrient delivery rates from foods using standardised in vitro methods calibrated against available in vivo data. This would give guidance to consumers on how rapidly they should expect various nutrient types to be released postprandially and could be backed up by public health information that explains the benefits of slow and steady nutrient release/absorption compared with the peaks and troughs that can be the result of rapid release/absorption.
The Glycemic Index (or Glycemic Load) of foods provides a carbohydrate-centred snapshot of the consequences of digesta dynamics and has broad appreciation at least in some countries where public health agencies have embraced the concept. As the measurement is an in vivo one, natural variation means that there is a challenge in achieving the same level of precision as can be achieved from laboratory analyses, so it is common for foods to be identified as low, medium or high GI to simplify communication. A similar approach could be used for not only carbohydrates but also other nutrients to identify slow, medium or fast release rates as an indicator of digesta dynamics.
Star ratings or similar quantitative amalgams of nutrition indicators are often dominated by nutrient composition and would also benefit from including digesta dynamics indicators, where these are available. The same argument applies to more qualitative food-level messaging such as traffic light symbols or health agency endorsements. In addition to current labelling practices that identify foods with high levels of e.g. fibre or protein, in the future labelling of slowly digested foods would be useful when sufficient data becomes available.
At this stage in the development of nutrition science, the in vivo data available on digesta dynamics is patchy and incomplete. However, the qualitative communication power of the concept can be exploited now. This would help to stimulate the technical challenge of developing an in vivo dataset that can be relied upon to provide quantitative guidance on digesta dynamics at the individual food or meal level. This challenge should not be underestimated as the measurements needed include gastric, small intestinal and large intestinal passage rates(Reference de Loubens, Capuano and Loverdo59) together with digestion and absorption rates of (at least) macronutrients across all regions of the digestive tract. If robust and sufficiently extensive in vivo data can be obtained, then in vitro digestion (and potentially absorption) models could be calibrated to generate predicted digesta dynamics. As with any set of in vivo measurements there will inevitably be not only inter-individual but also intra-individual variations that will need to be understood(Reference Ni, Smyth and Cozzolino60). The advantage of knowing this is twofold. First, the accuracy of any predicted in vitro measure can be appreciated, and secondly inter-individual differences can be used to inform personalised nutrition advice. Notwithstanding the inevitable uncertainty from in vivo data, it is a reasonable expectation that results should show how individual foods are ranked in terms of their digesta dynamics.
The in vivo measurement of parameters that can be used to characterise digesta dynamics is challenging but, with sufficient resources and focus, should be possible. For a test food, there are three types of connected information that are useful: (i) timescales of residence/passage through the stomach, small intestine, large intestine, linked with (ii) molecular composition and residual digesta particle architecture at each relevant site and (iii) time courses of nutrient contents in the blood as an indicator of absorption. The first two of these are very difficult to achieve currently and will require the innovative use of imaging, sampling and labelling approaches as discussed below. The sampling of blood is straightforward and could encompass hormonal signals as well as absorbed nutrients, but active metabolism needs to be considered. Sophisticated non-invasive blood analyses are now possible using skin patches as widely used to monitor e.g. glucose excursions in real time(Reference Metwally, Heydari and McDuff61). Extension of the technology to additional nutrients of interest could generate datasets both in real time and for enough people to provide meaningful statistics.
Measurement of passage rates through the various segments of the digestive tract requires the use of non-digested markers and is well established for model species such as pigs(Reference Low, Pluschke and Gerrits62,Reference Low, Pluschke and Flanagan63) . However, this involves invasive studies that are not applicable to humans, so alternative methods are needed. Combinations of imaging techniques (potentially via both external methods(Reference Deng, Le Feunteun and Diascorn64) and swallowed cameras) and digesta capture from e.g. site-specific triggered capsules(Reference Shalon, Culver and Grembi65) could in principle provide the relevant information, but major resolution and species detection challenges will need to be resolved for imaging techniques and representative digesta capture will need to be achieved from triggered capsule devices. In previous decades, the key measure of time to the end of the small intestine and nutrient content entering the large intestine was estimated from ileostomy subjects whose digesta flows to an external pouch following surgery to treat a diseased or malfunctioning large intestine. Whilst this could continue to be a valuable source of information, it is now understood that fermentation and metabolite absorption in an intact large intestine generates systemic hormonal and other signals that influence digesta passage(Reference Dagbasi, Cai and Hirdaramani47,Reference Cherbut, Aube and Blottiere66) .
The current lack of routine methods for quantifying digesta transit times and nutrient release rates means that digesta dynamics is not yet ready to form the basis for food classification. However, the mechanistically sound relationships between parameters of passage and/or nutrient absorption timescales and NCD risks means that their use for food classification purposes is worth pursuing. In contrast, there is no persuasive mechanism that explains why only UPFs as opposed to a broader range of processed foods contribute to NCD risks. If UPF status is used to classify foods as ‘unhealthy’, there will have to be a means of analysing foods (without knowing their processing history) to determine whether they fall into the UPF category or not. Whatever technical criteria or analysable components are used, a foreseeable consequence is that food manufacturers will reformulate their products so that they do not fall into the UPF category. This will both reduce the credibility of the UPF message and do nothing to address the real NCD risks from many processed foods that are due to nutrient contents and digesta dynamics not food additives.
Conclusion
Digesta dynamics may not be ready to form the basis for food classification yet but could play a useful role in explaining why many UPFs and other processed/assembled foods are associated with increased NCD risk. Greater awareness of the timescales of passage, digestion, fermentation and absorption as a result of different food choices should be pursued through nutrition communication today. Future research on digesta dynamics should identify quantitative features that can be used to (i) develop robust and calibrated in vitro models and (ii) provide information for food labelling and classification in the future.
Acknowledgements
None.
Author contribution
MJG is the sole author of this manuscript.
Financial support
No external financial support to declare.
Competing interests
The author declares that there are no conflicts of interest associated with this review.

 Open access

