Implications
Seasonality of reproduction in sheep has a genetic component; however, the results of classical polygenic selection for the traits associated with spring breeding are limited. The use of polymorphic quantative trait loci or associated genetic markers could improve the efficiency of selection. Various studies on different sheep breeds suggest that polymorphism in the MT1 receptor gene may be a potential marker of selection. This study of Merinos ewes, tests the linkage between this polymorphism and the expression of seasonality. The results do not support the use of genotyping for MT1 as a means of selection for aseasonality.
Introduction
Seasonality of reproduction remains an important constraint in temperate sheep breeds in which ovulatory activity generally is inhibited in spring. Measurements of spontaneous ovulatory activity (SOA) in early spring, before the introduction of males into the flock, has been used to study out-of-season breeding ability in several low seasonal sheep breeds such as Merinos d’Arles (MA; Hanocq et al., Reference Hanocq, Bodin, Thimonier, Teyssier, Malpaux and Chemineau1999), Latxa (Beltran de Heredia et al., Reference Beltran de Heredia, Urgate, Malpaux, Canepa and Bodin2002) and Chios (Avdi et al., Reference Avdi, Banos, Kouttos, Bodin and Chemineau2003). Very similar results with regard to SOA have been found in the above studies; this trait is repeatable and its heritability ranges from 0.12 to 0.22. In the MA breed, a strong association has been observed between breeding value for SOA in April and restriction polymorphism at position 605 in Exon II of the MT1 melatonin receptor gene, corresponding to the presence (allele +) or absence (allele −) of a MnlI restriction site (Pelletier et al., Reference Pelletier, Bodin, Hanocq, Malpaux, Teyssier, Thimonier and Chemineau2000). More intense seasonality was associated with genotype −/−. The discovery of this association extended previous results of Messer et al. (Reference Messer, Wang, Tuggle, Yerle, Chardon, Pomp, Womack, Barendse, Crawford, Notter and Rothschild1997) and could point to a specific role of the MT1 genotype in seasonal anoestrus; this study was designed to test this hypothesis. After genotyping MA ewes in a single flock in the first year of the study, groups of ewes from each homozygous genotype (+/+ and −/−) were identified and their SOA was assessed between the end of drying-off (January) and the beginning of spring mating (April) over two consecutive years. In the first year of this observation period (year two of the study), groups of ewes were managed together on rangelands (experiment 1). In the following year, they were kept in a sheepfold where half of the ewes of each genotype were fed at a higher level than the other half to also test the effect of feeding levels on SOA (experiment 2). This study provides results on genotype frequencies in MA, on SOA in early April for the genotyped ewes, and on the follow-up of SOA of +/+ ewes and −/− ewes between January and mid-April (before spring mating) under different experimental conditions.
Material and methods
Association study between genotype at the MnlI locus and SOA
Following genotyping of 314 MA ewes for the MnlI site early in 2003, their SOA was assessed in April of two consecutive years (2003 and 2004) by measuring peripheral progesterone levels twice in a 9-day period. These ewes from one flock belonging to an experimental farm, Le Merle (south-eastern France, latitude 43.5°N), were born in autumn lambing from 1998 to 2001, that is, aged 1 to 4 years at the beginning of 2003. The flock was established in the 1920s and at the time of the study included approximately 1100 pure MA ewes and 30 rams. Renewal was about 20% per year and the foreign breeding material introduced, consisting only of rams or semen, came from a regional breeding centre where male lambs from different sheep flocks were raised to provide breeding rams. These rams were the offspring of ewes qualified as ‘ram dams’ whose selection criteria were unrelated to seasonality with the exception that the male lambs had to be born in autumn to enter the breeding centre. Over the last 14 years, the percentage of ewes from identified sires has remained above 50%. Genotyping was performed on 314 DNA samples prepared from ewes using the procedure described in detail by Pelletier et al. (Reference Pelletier, Bodin, Hanocq, Malpaux, Teyssier, Thimonier and Chemineau2000). The resulting genotypes were represented as +/+, +/− and −/− according to the presence (allele +) or absence (allele −) of the MnlI restriction site. In addition, the physiological status for SOA of the genotyped ewes (anovulatory or ovulatory) was determined in early April for 2 years (2003 and 2004). For this, we used the criteria established by Thimonier (Reference Thimonier2000), which hold that plasma progesterone concentrations in two blood samples taken 7 to 11 days apart are adequate for the detection of ovulatory activity at a given period in ewes with regular ovarian cycles of 17 days on average and to discriminate the two physiological statuses. The most accurate results are obtained at an interval of 9 days between blood samples. Out of the 314 genotyped ewes, 312 were sampled twice in April 2003; however, only 289 were sampled in April 2004 because some had died or had been culled over the intervening year. Ewes with a progesterone level above the threshold of 1 ng/ml in at least one of the two consecutive blood samples were considered to be ovulatory or cycling. Progesterone concentrations were measured by radio-immunoassay using the technique described by Terqui and Thimonier (Reference Terqui and Thimonier1974).
As a rule, all of the MA ewes involved in the study were mated for the first time at 18 months of age and were joined with rams between April and June in subsequent years. They were kept completely separate from males during the months between the annual spring mating.
Assessment of SOA over a long period in +/+ and −/− ewes
Experiment 1
In early 2004, two groups of 30 +/+ and 30 −/− ewes of similar age distribution (2, 3 and 5 years old) were identified from the population of genotyped ewes. The other sampling criteria for adults (3 and 5 years old) were fertility and the number of lambs suckled during the previous autumn lambing. The paternity of all of the ewes was not known; however, when possible, we tried to include ewes from different sires. From 15 January to 14 April, the SOA of ewes was assessed by measuring progesterone concentrations in blood samples taken 7 days apart. As the period of observation was long, the 7-day interval was chosen for logistical reasons, that is, to have a fixed day each week to take blood samples in the ewe groups. With this collection interval, the detection of ovulation is similar to that obtained with an interval of 9 days, especially when one can examine the progesterone levels in more than two consecutive blood samples to determine the status of SOA at a given period (Thimonier, Reference Thimonier2000). The ewes were kept on separate rangelands to avoid repeated sorting of animals during the experiment, and their shearing was carried out over a single day at the end of March. At the end of blood sampling, the two groups of ewes were reunited on 15 April and three rams were introduced into this combined group for 1 month. They then joined the rest of the spring mating MA flock from mid-May to mid-June.
Experiment 2
In January of the following year (2005), 60 ewes from the population of genotyped ewes were divided into two groups of 30 ewes each; in each group, 15 ewes were +/+ and 15 ewes were −/−. These groups of ewes of similar age distribution (3, 4 and 6 years old) were balanced in terms of live weight (LW), body condition score (BCS), fertility and the number of lambs suckled during the previous autumn lambing. Several ewes involved in this experiment (15 +/+ and 7 −/−) were not the same as in the previous year due to the sampling procedure and the replacement of dead or culled animals. The two groups of ewes were transferred to a sheepfold with natural light and, after a 15-day period of acclimatization together, placed in two adjacent pens with different feeding levels from 3 February to 14 April. One group was fed at a low level (L): 70% of maintenance energy requirements, with a diet composed of straw and pelleted alfalfa. The other one was fed at a high level (H): about 170% of maintenance energy through the addition of pelleted alfalfa and pelleted beet pulp. Daily rations for the H and L diets were formulated to increase the BCS by about 1 point in 60 days (H diet) or to maintain the LW and BCS at the level at which they were at the end of drying-off (L diet). The H diet was reduced to maintenance requirements beginning in late March to prevent excessive fattening at mating. Daily rations were established on the basis of standard feeding values for the ingredients (Jarrige, Reference Jarrige1988). They were distributed, between midday and 1400 h, in racks allowing simultaneous access to all ewes. In each pen, the ewes had free access to water, salt blocks and a mineral–vitamin pre-mix.
Immediately before the different diets were introduced, SOA was determined by the progesterone levels in the two blood samples taken 9 days apart, using the rules of interpretation already defined for the two samples. SOA was then assessed through blood samples collected at 9- to 10-day intervals from 25 February to 14 April. Ewes were weighed at this interval and their condition scored at a double interval on a 5-point graded scale (Russel et al., Reference Russel, Doney and Gunn1969) with 0.25 subdivisions. After an additional 12-day period of re-feeding (or feeding) at the maintenance requirement level in the sheepfold, the ewes were exposed to rams on pastures from 27 April to mid-June. For this experiment, shearing was delayed until the beginning of May, that is, during the mating period.
Periods of SOA
For the long-term experiments, determination of status (cycled or non-cycled) of a ewe at each blood sampling point of time was based on progesterone level at the time of sampling and additional information obtained from other progesterone measurements on the same ewe during the sampling period. Unlike the analysis of two consecutive blood samplings, interpretation of progesterone levels in sequential blood samples required taking into account the timing of observations. A measurement below the threshold of 1 ng/ml of progesterone (coded 0, non-cyclic or follicular phase) that followed a measurement above the threshold (coded 1, luteal phase) was therefore included systematically in the definition of periods of SOA. With the 7-day interval retained in experiment 1, the infrequent occurrence of two consecutive measurements below the threshold that both followed and preceded observations above the threshold also were included in periods of continuous activity. For example, in experiment 1, the vector of n observations for a ewe [1 0 1 1 0 0 1 0 0 0 0 1 1 0] was interpreted as [ 1 1 1 1 1 1 1 0 0 0 1 1 1]. In experiment 2, in which blood samples were taken 9 or 10 days apart, the vector [0 1 0 1 0 0] was interpreted as [ 1 1 1 1 0]. The first observation was used to determine the SOA of ewes at the following date and analysis of modified data was carried out on n−1 variables.
Statistical procedures
The repeatability of SOA for the 2 years of measurements in April on all genotyped ewes was estimated by the coefficient φ, which is a measure of the degree of association between all-or-nothing traits as two binary variables (Yule, Reference Yule1912).
The effects of genotype and feeding level on SOA variables (0/1 modified data) were investigated by a logistic regression of longitudinal data sets from experiments 1 and 2 using a marginal model, generalized estimating equations (GEE; Diggle et al., Reference Diggle, Heagerty, Liang and Zeger2002). GEE can be regarded as an extension of GLM for the analysis of correlated data. In the general framework of longitudinal analysis, GEE takes into account the dependency of repeated observations within subjects by specifying a ‘working correlation structure’. In this case, the correction for within-ewe correlation was carried out by assuming an auto-regressive correlation structure for the repeated-in-time measurements. This option was retained in the model to obtain efficient estimates of the standard error (robust s.e.) of coefficients and hence efficient inference tests (Wald test), the Wald statistic being used for assessing significance of coefficients (Hosmer and Lemeshow, Reference Hosmer and Lemeshow2000). Under the null hypothesis, this statistic, also called z, will follow a standard normal distribution.
In these analyses, the date of observation was introduced as a linear continuous variable (coded from 0 for the first date to n for the last date) and genotype, age and diet as categorical variables. Interactions that are important for interpreting the effect of genotype, for example, genotype by date and genotype by diet, were introduced in a first step and were excluded from the final model if they had no significant effect (Wald test with a P-value >0.05). The genotype −/−, the first class of age (2 or 3 years old according to the studied data set) and the L diet were used as reference categories. Analyses were performed using R software: GEE function, binomial family, logit link, AR-M (M = 1) correlation structure (R Development Core Team, 2007).
Other comparisons between genotypes (and feeding levels) on SOA percentage were carried out using χ 2 test and odds ratio (OR, and CI for its confidence interval). One-tailed t-test was used for the comparisons between feeding levels on ewe LW and ewe BCS.
Results
Genotypic frequencies and SOA in April
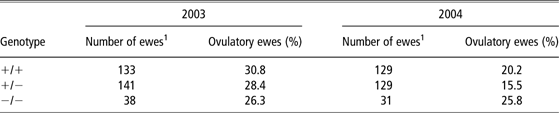
Frequencies of genotypes +/+, +/− and −/− in the population of 314 genotyped ewes were 43.0% (n = 135), 44.9% (n = 141) and 12.1% (n = 38), respectively; this agrees with the Hardy–Weinberg equilibrium (p 2, 2pq, q 2 with p = 0.65 and q = 1−p) and suggests that the MnlI locus is not under selection in the MA population under investigation. With regard to this large sample of MA ewes (Table 1), there was no significant difference between genotypes in the percentage of ovulatory ewes in early April in either year of measurement (χ 2 test: P = 0.83 and P = 0.35 in 2003 and 2004, respectively). Only 30 ewes were ovulating in early April in both of the 2 years, and none was of genotype −/− (17 +/+, 13 +/−). The repeatability of SOA for the two consecutive years was 0.28.
Percentage of ovulatory ewes in early April in the MA genotyped for the MnlI site, according to genotype and year of measurement

MA = Merinos d’Arles.
1Number of ewes sampled on 2 and 11 April 2003 (n = 312); 5 and 14 April 2004 (n = 289).
Time changes in SOA of homozygous ewes
Experiment 1
Two ewes of genotype −/− were eliminated during the experiment: one at the beginning, the other died before the last blood sampling. The representation of changes in the percentage of cyclic ewes from January to mid-April (Figure 1) displays a similar change in SOA over time in both groups of ewes (30 +/+ and 29 to 28 −/−). This change was marked by the occurrence of a temporary rise in ovulatory activity triggered prior to shearing on 29 March. In early April, which is the usual period of SOA measurement before rams are introduced, no difference was observed between genotypes. The overall percentage of cyclic ewes on 14 April was 25.9%.
Changes in the percentage of cyclic ewes between January and mid-April for +/+ ewes (n = 30) and −/− ewes (n = 29 to 28) in experiment 1.

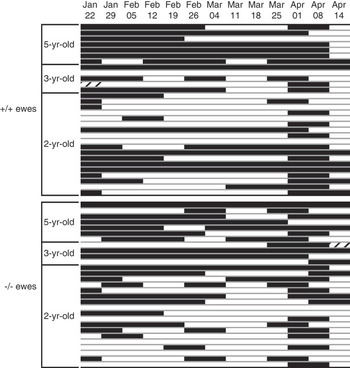
Patterns of SOA for individual ewes (Figure 2) show that many ewes of both genotypes exhibited discontinuities in their ovulatory activity. In several of these ewes, no ovulatory activity was detected for periods of 2 to 3 weeks, suggesting the failure of a single cycle. The proportion of ewes continuously cycling at least until the apparent end of their SOA (11/30 and 6/29 for ++ and −/− ewes, respectively) did not differ significantly between genotypes (OR = 2.22 with a 95% CI of 0.69, 7.12).
Periods of spontaneous ovulatory activity for individual ewes in experiment 1 sorted by age within genotype. Hatched areas indicate the absence of observation, open areas indicate periods of anovulatory activity.

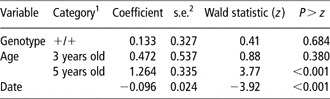
The results of the GEE analysis of this data set showed in the first place that the interaction between genotype and date was not significant. Therefore, the final fitted model was reduced to the main effects of genotype, age and date variables (Table 2). The effect of genotype on SOA was not significant (P = 0.68). For the age effect, the 5-year-old ewes were much more likely to be cyclic than the 2-year-olds (P < 0.001), while no significant difference was observed between 3- and 2-year-old ewes (P = 0.38). The effect of date was highly significant (P < 0.001) with a negative estimate of the coefficient; this linear variable indicates an overall decrease of SOA among the ewes from January to mid-April.
Estimated coefficients, s.e., Wald statistics and P-values for the GEE model fitted to SOA data set from experiment 1, including genotype and age categorical variables and date continuous variable

GEE = generalized estimating equations; SOA = spontaneous ovulatory activity.
1Reference categories for categorical variables are not included.
2Robust s.e. of the coefficients provided by the GEE method with the option of an auto-regressive structure of correlation within each ewe.
z = coefficient/s.e., with P-value calculated from a normal table.
Experiment 2
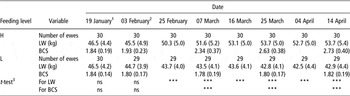
Changes in ewe LW and ewe BCS during this experiment are shown in Table 3 for the groups of ewes fed at high and low levels (15 or 14 +/+ and 15 −/− ewes per group; one +/+ ewe was eliminated early after the constitution of the ewe groups). Average values for LW and BCS, which were equal between groups when they were constituted, differed significantly after 1 month of differential diets. From early February until the end of the experiment, the H diet induced an increase of 8.2 kg for LW and 0.8 point for BCS, while these traits remained approximately constant until the end of experiment for the ewes on the L diet.
Evolution of LW and BCS in the groups of ewes fed at H and L levels (170% and 70% of maintenance energy requirements, respectively) from early February: mean value (s.d.)

LW = live weight; BCS = body condition score; H = high level; L = low level.
1Constitution of the groups of ewes.
2Start of differential feeding levels.
3Unilateral t-test by the hypothesis that the mean value for H diet was greater than the mean value for L diet.
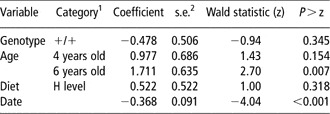
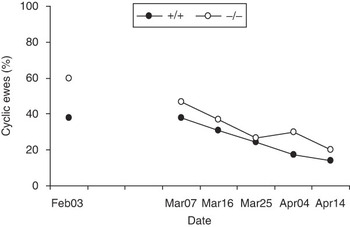
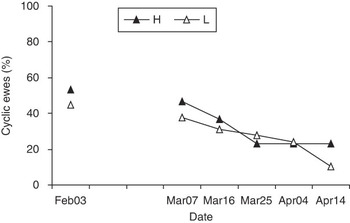
For this controlled group feeding experiment, results of the GEE analysis of the SOA data set from 7 March to mid-April, when the ewes had been fed at different levels since early February, indicated similar trends as in experiment 1. The interaction between genotype and date as well as between genotype and diet were not significant; they consequently were excluded from the final model whose results are given in Table 4. These results confirmed the absence of effect of genotype on SOA (P = 0.35); the presence of effect of age, with the 6-year-old ewes significantly more cyclic than the 3-year-olds (P < 0.01); and the significant decrease in SOA among ewes during the period of study (P < 0.001). In addition, the result for the diet variable (P = 0.32) showed that the feeding level had no significant effect on the cyclicity of ewes within this period. The corresponding changes in SOA according to genotype (irrespective of diet) or to diet (irrespective of genotype) are presented in Figures 3 and 4, respectively. At the end of this experiment on 14 April, the average percentage of cyclic ewes was 16.9%.
Estimated coefficients, s.e., Wald statistics and P-values for the GEE model fitted to SOA data set from experiment 2 (7 March to 14 April), including genotype, age and diet categorical variables and date continuous variable

GEE = generalized estimating equations; SOA = spontaneous ovulatory activity; H = high level.
1Reference categories for categorical variables are not included.
2Robust s.e. of the coefficients provided by the GEE method with the option of an auto-regressive structure of correlation within each ewe.
z = Coefficient/s.e. with P-value calculated from a normal table.
Changes in the percentage of cyclic ewes between February and mid-April for +/+ ewes (n = 29) and −/− ewes (n = 30) in experiment 2 (irrespective of diet).

Changes in the percentage of cyclic ewes between February and mid-April for H level (n = 30) and L level (n = 29) ewes in experiment 2 (irrespective of genotype). Ewes were fed at different levels from 3 February.

Fertility in spring mating
In experiment 1, in which ewes were joined with rams the day after the last blood sampling, there was no significant difference between genotypes in fertility in spring mating: 90% of +/+ ewes and 89.3% of −/− ewes later lambed the following autumn. There also was no difference in prolificacy (1.32 and 1.28, respectively). During the first 15 days after joining, on the basis of autumn lambing, there were a few more +/+ ewes fertilized or conceiving than −/− ewes (6 and 3 ewes, respectively), but this difference was not significant. Furthermore, the cumulative distribution of lambing dates did not differ significantly between genotypes (P > 0.05, non-parametric Kolmogorov–Smirnov two-sample test). In experiment 2, the comparison between genotypes of the fertility of ewes after the spring mating was not an objective because of the 12-day period of re-feeding of underfed ewes before mating and the delayed shearing time, which had been postponed until after mating began.
Discussion
Pelletier et al. (Reference Pelletier, Bodin, Hanocq, Malpaux, Teyssier, Thimonier and Chemineau2000) have shown that a mutation at position 612 in Exon II of the ovine MT1 gene leads to the absence of a cleavage site for the MnlI enzyme at position 605 (allele −). They showed that this mutation was always found to be associated with a single allelic isoform among the different isoforms described for this exon. This haplotype is characterised by the specific and constant presence of four mutations, including the one (612) responsible for MnlI polymorphism, two other silent mutations at positions 453 and 891, and a mutation at position 706 that results in one base change in the amino acid sequence of the predicted MT1 receptor protein (substitution of a valine by an isoleucine). Several independent results point out a potential functional role of this locus on the control of seasonality:
1. Within breeds, Pelletier et al. (Reference Pelletier, Bodin, Hanocq, Malpaux, Teyssier, Thimonier and Chemineau2000) found a highly significant difference in the frequency of homozygotes −/− between two groups of MA ewes screened for their SOA in spring. Ewes homozygous for the absence of the MnlI site were not observed in the group of ewes cycling in April over three consecutive years (1995 to 1997). This study conducted on the same flock showed that −/− ewes also were not found in the group of 30 ewes that cycled in April over two consecutive years (2003 and 2004). Furthermore, a significant effect of MnlI polymorphism on fertility in spring mating has been reported (Notter et al., Reference Notter, Cockett and Hadfield2003) for adult ewes from a composite line (50% Dorset, 25% Rambouillet, 25% Finnsheep). Adult ewes with the genotype −/− had lower spring fertility. Significant differences between +/+ or +/−, and −/− genotypes in lambing frequency also were reported among Dorset ewes managed by an accelerated lambing system (Mateescu et al., Reference Mateescu, Lunsford and Thonney2009).
2. Comparisons between breeds also support the functional role of the MT1 genotype. Substantial changes in allelic frequencies at the MnlI site with the degree of seasonality of breeds have been described by several different authors (Messer et al. Reference Messer, Wang, Tuggle, Yerle, Chardon, Pomp, Womack, Barendse, Crawford, Notter and Rothschild1997; Pelletier et al. Reference Pelletier, Bodin, Hanocq, Malpaux, Teyssier, Thimonier and Chemineau2000; Notter and Cockett, Reference Notter and Cockett2005). For example, ewes of seasonal breeds had relatively higher frequencies of genotype −/− than ewes of low seasonal breeds. Thus, genotype −/− was not found in a large sample of ewes from the non-seasonal small-tailed Han breed in China (Chu et al., Reference Chu, Ji and Chen2003) and the following gradient of the percentage of −/− ewes was encountered in samples of several breeds: 9% in Blackbelly; 7% in Barbarine; 10% in MA; 31% in Ile-de-France; 35% in Suffolk; 100% in wild Mouflon (Trecherel, Reference Trecherel2007).
3. Various physiological studies reinforce the assumption of a close relationship between the expression of seasonality and polymorphism of the MT1 receptor gene. In MA −/− ewes, a higher density of melatonin receptors has been found in the pars tuberalis (Pelletier et al., Reference Pelletier, Bodin, Hanocq, Malpaux, Teyssier, Thimonier and Chemineau2000) as well as in four other brain areas (Trecherel, Reference Trecherel2007). One of these areas belongs to the pre-mammillary hypothalamus, which is an important site of melatonin action regulating the reproductive function in sheep (Malpaux et al., Reference Malpaux, Migaud, Tricoire and Chemineau2001).
4. Moreover, the contrast between the unique allelic isoform of Exon II associated with higher seasonality in several breeds and large variability of other haplotypes suggests a common origin of this particular haplotype, which had not been lost through selection and dissemination due to the selective advantage it confers.
Despite these findings, the relationship between the studied part of Exon II of the MT1 gene and the phenotype of seasonality remains unclear. First, this study indicates that in MA, no difference was observed between ewes of genotype +/+ and −/− in the rate of SOA in early spring or on fertility in spring mating. Second, various attempts failed to find a difference by various criteria (beginning, end or length of the breeding season) within the genotyped progeny (+/+ and −/−) of heterozygous sires in Ile-de-France (Hernandez et al., Reference Hernandez, Bodin, Chesneau, Guillaume, Chemineau, Malpaux and Migaud2005) and Latxa breeds (Ugarte et al., Reference Ugarte, Beltran de Heredia and Bodin2007).
How may these two contradictory sets of findings be reconciled? It is unlikely that the relationship between the expression of seasonality and polymorphism of the MT1 gene found in MA (Pelletier et al, Reference Pelletier, Bodin, Hanocq, Malpaux, Teyssier, Thimonier and Chemineau2000), OOS (Notter et al., Reference Notter, Cockett and Hadfield2003) and Dorset (Mateescu et al., Reference Mateescu, Lunsford and Thonney2009) ewes is casual. On the other hand, the mutated haplotype has been observed in enough animals of different breeds to exclude a sampling artefact. One hypothesis explaining this discrepancy would be the existence of another non-conservative mutation on an independent gene. Selection for spring ovulation would increase the frequency of favourable alleles at both sites, including the MnlI site. This would explain the results observed by Pelletier et al. (Reference Pelletier, Bodin, Hanocq, Malpaux, Teyssier, Thimonier and Chemineau2000). In contrast, the screening of animals only for the presence or absence of the MnlI site would not have any influence on the proportions of alleles at the other site, and this therefore would be insufficient to induce a change in the expression of seasonality. Support for this hypothesis would come when such a non-conservative mutation has been identified; however, it has not yet been found.
With regard to environmental effects, it is important to note that the beginning of the unexpected rise of SOA in the first experiment (experiment 1) was observed on 25 March, that is, 4 days before shearing. No other change in management, handling or treatment may be associated with the increase of SOA on this date. The amplitude of the peak of SOA was probably related to shearing; however, its start before shearing might reflect spontaneous changes in the Mediterranean environment of grazing ewes with an increase in pasture availability and forage intake on rangelands after the colder months (January and February). Such events (shearing, re-growth on rangelands) could partially explain the inter-annual variations of the cyclicity rate observed in early April for MA ewes from first generations of selection lines for SOA at this time (Teyssier et al., Reference Teyssier, Canepa, Chemineau, Malpaux, Migaud and Bodin2002). The introduction of controlled feeding levels in experiment 2 was also justified by different studies that have shown relationships between ovulatory activity and LW and BCS of ewes from Merino flocks (Hanocq et al., Reference Hanocq, Bodin, Thimonier, Teyssier, Malpaux and Chemineau1999; Kleemann and Walker, Reference Kleemann and Walker2005). In this study, the occurrence of a small divergence between diets at the end of the study period might suggest a delayed effect of feeding level on SOA (Teyssier et al., Reference Teyssier, Migaud, Debus, Maton, Bouquet, Bocquier, Chemineau, Malpaux and Bodin2006), but such a hypothesis was clearly challenged by the final analysis of results using a model suited to this type of data. The substantial differences in LW and BCS induced by differential feeding levels from February thus had no significant effect on SOA at the beginning of April. This agrees with results on Barbarine ewes (Khaldi, Reference Khaldi1984), which have shown that significant variations of ewe LW between drying-off and the spring introduction of rams had no significant effect on the percentage of cyclic ewes before the beginning of mating, whereas initial differences in LW established during a pre-experimental period before drying-off significantly affected this percentage.
In conclusion, results of this study show that genotype at locus MnlI of the MT1 receptor gene cannot be used alone as a genetic selection marker for spring (out-of-season) breeding in sheep, at least not in the MA breed. Further studies are required to define the role of this genomic region in the expression of seasonality. In addition, while the results illustrate the responsiveness of SOA to events such as shearing and spontaneous variations in the Mediterranean environment of grazing ewes, they do not show a significant effect of differential feeding of sheepfold ewes after drying-off on their SOA before spring mating.
Acknowledgements
We wish to thank especially P.M. Bouquet in charge of the experimental farm ‘Domaine du Merle’, J.D. Guyonneau, D. Montier and J.M. Capron for their contribution to the experiments and the staff of the INRA assay laboratory of Nouzilly for the progesterone assays. We are also grateful to A. Collet who performed genotyping of ewes. This work was supported by Institut National de la Recherche Agronomique (INRA): Departement PHASE (Grants CI 2004 and CI 2005), Departement GA.