


INTRODUCTION
Diplozoinae contains 5 genera, i.e. Diplozoon Nordmann, 1832, ParadiplozoonAchmerov, Reference Achmerov1974, InustiatusKhotenovsky, Reference Khotenovsky1978, SindiplozoonKhotenovsky, Reference Khotenovsky1981 and EudiplozoonKhotenovsky, Reference Khotenovsky1985 (Achmerov, Reference Achmerov1974; Khotenovsky, Reference Khotenovsky1978, Reference Khotenovsky1981, Reference Khotenovsky1985). The phylogenetic relationship of diplozoids has been examined only in several species occurring in Europe (Matejusová et al. Reference Matejusová, Koubková, D'amelio and Cunningham2001; Sicard et al. Reference Sicard, Desmarais and Lambert2001). Despite this, little is known about the relationship among the 5 genera of diplozoids.
Khotenovsky (Reference Khotenovsky1985) listed 43 species belonging to the Diplozoinae and 6 species inquirenda from former Soviet Union. In Europe, there are about 18 species belonging to 2 genera, Diplozoon and Paradiplozoon in the Diplozoinae (Matejusová et al. Reference Matejusová, Koubková and Cunningham2004), and the occurrence of Eudiplozoon nipponicum in Europe is considered as introduced from Asia (Denis et al. Reference Denis, Gabrion and Lambert1983). In China, a total of 31 species belonging to 4 genera, i.e. 22 in Paradiplozoon, 6 Sindiplozoon, 2 Inustiatus and 1 Eudiplozoon in the Diplozoinae has been summarized (Wu et al. Reference Wu, Long and Wang2000), of which only 9 have been reported by Khotenovsky (Reference Khotenovsky1985).
Molecular markers may also provide information useful for the discrimination of diplozoids, as the determination of species within some genera is difficult and relies only on the measurement of the central hook, and clamp (Khotenovsky, Reference Khotenovsky1985). Moreover, measurements of those morphological characteristics may be variable even within species and are considered unreliable for species identification (Gläser and Gläser, Reference Gläser and Gläser1964; Matejusová et al. Reference Matejusová, Koubková, Gelnar and Cunningham2002). The nucleic acid sequence of the second internal transcribed spacer of ribosomal DNA (ITS-2 rDNA) has been suggested to be a powerful tool for the separation of species in Diplozoon and Paradiplozoon (Matejusová et al. Reference Matejusová, Koubková, D'amelio and Cunningham2001, Reference Matejusová, Koubková and Cunningham2004; Sicard et al. Reference Sicard, Desmarais and Lambert2001). However, there are indeed different views in respect to the identification of some species in Diplozoon and Paradiplozoon. Paradiplozoon, which was initially created as a subgenus in Diplozoon according to morphological differences mainly in the central part of the posterior body part (Achmerov, Reference Achmerov1974), was raised to the genus status by Khotenovsky (Reference Khotenovsky1981), and more than 20 species were moved to the Paradiplozoon, with only 2 species remaining in the Diplozoon, i.e. D. paradoxum and D. scardinii (Khotenovsky, Reference Khotenovsky1985). However, Le Brun et al. (Reference Le Brun, Renaud and Lambert1988) and Sicard et al. (Reference Sicard, Desmarais and Lambert2001) used the genus status Diplozoon for all representatives of diplozoids in their research, so in fact Diplozoon homoion and D. bliccae are synonymous to Paradiplozoon homoion and P. bliccae in other studies. Using ITS2 and LSU rDNA sequences, Sicard et al. (Reference Sicard, Desmarais and Lambert2001) found that D. scardinii, considered as a specific parasite of Scardinius erythrophthalmus, is identical to Paradiplozoon homoion from Rutilus rutilus, leaving only 1 species, D. paradoxum, in the genus Diplozoon.
The present study aimed to investigate the molecular phylogenetic relationship among all 5 genera in the Diplozoinae. Species in Paradiplozoon, Eudiplozoon, Inustiatus and Sindiplozoon, which occur on freshwater fish in China, were collected for sequencing the ITS-2 rDNA. In addition, all published ITS-2 rDNA data for diplozoids, including species in the genera Diplozoon, Paradiplozoon, and Eudiplozoon were incorporated in the phylogenetic analysis.
MATERIALS AND METHODS
Collection of parasites
A total of 9 formerly described diplozoid species was collected from gills of 11 species of cyprinid fish from three lakes and one reservoir in China (Table 1). Parasites were removed from the gills under a dissecting microscope, and identified under a light microscope according to the description by Khotenovsky (Reference Khotenovsky1985) and Wu et al. (Reference Wu, Long and Wang2000). Specimens were washed in double-distilled water before being fixed in 90% ethanol for molecular analysis.
List of diplozoid species used in this study with host species, locality of collection and GenBank Accession number
(Asterisks indicate species sequenced in this study.)

Note: 1. Species names of European diplozoids listed in this table are those found in the GenBank, and some are synonymous: D. bliccae and D. homoion are synonymous to P. bliccae and P. homoion, respectively.
2. The number following species names representing samples either from different host species or from different localities.
Sequencing of the second internal transcribed spacer of ribosomal DNA (ITS-2 rDNA)
Ethanol-fixed parasites were soaked for 1 day in TE buffer (pH 8·0) to remove ethanol, and the genomic DNA was extracted from individual specimens using a standard SDS-proteinase K procedure as described by Sambrook et al. (Reference Sambrook, Fritsch and Maniatis1989). The DNA was ethanol-precipitated and resuspended in 30 μl of distilled water. Universal eukaryotic primers, D (5′ GGCTYRYGGNGTCGATGAAGAACGCAG 3′) and B1 (5′ GCCGGATCCGAATCCTGGTTAGTTTCTTTTCCT 3′) (Bachellerie and Qu, Reference Bachellerie, Qu and Hyde1993), were used to amplify the ITS-2 rDNA region. PCR amplification reaction was performed in a 100 μl vol. containing 4 μl of DNA template, 5 μl of 10×PCR buffer (TaKaRa), 200 μm of each dNTP, 0·5 μm of each primer, 1·25 units of Taq polymerase (TaKaRa), under the following conditions: 10 min at 95°C, 30 cycles of 30 sec at 95°C, 30 sec at 65°C and 75 sec at 72°C, followed by a final elongation of 10 min at 72°C. Samples without genomic DNA (control) were included in each amplification run. PCR products were detected on ethidium bromide-stained 1% agarose gels, and then purified from agarose gels. Purified products were cloned into pGEM-T vector (Promega, USA) and both strands were sequenced using an ABI BigDye Terminator V3.1 Cycle Sequencing Kit (E. Z. N. A.® Gel Extraction Kit; Product No. D2501-02, Omega) and ABI Cycle Sequencer 3700 (Foster City, CA, USA), and using M13+ and M13− primers. Sequences obtained were deposited in the GenBank database with Accession numbers listed in Table 1.
Sequence alignment and phylogenetic analysis
A total of 29 ITS-2 sequences were aligned automatically using Clustal X (1.8) with default gaps and weighing values (Thompson et al. Reference Thompson, Gibson, Plewniak, Jeanmougin and Higgins1997) and improved manually using SEAVIEW (Galtier et al. Reference Galtier, Gouy and Gautier1996). Accession numbers of diplozoid species retrieved from the GenBank database used in the alignment, their host species and sampling localities are given in Table 1. The outgroup Neoheterobothrium hirame belonging to the Diclidophoridae was also extracted from the GenBank database (Accession no. AB162613) and was used to root trees.
Base composition data and nucleotide substitutions between pairwise distances were generated using MEGA version 2.1 (Kumar et al. Reference Kumar, Tamura, Jakobsen and Nei2001) and DAMBE version 4.2 (Xia and Xie, Reference Xia and Xie2001).
Three different methods, i.e. neighbour-joining (NJ) and maximum likelihood (ML) in PAUP*4.0b10 (Swofford, Reference Swofford2003) and a Bayesian approach as implemented in MrBayes 3.0b (Huelsenbeck and Ronquist, Reference Huelsenbeck and Ronquist2001), were used to perform the phylogenetic analyses. The most appropriate evolutionary model GTR+G model (Gu et al. Reference Gu, Fu and Li1995) selected by AIC as implemented in MODELTEST 3.7 (Posada and Crandall, Reference Posada and Crandall1998) was used to construct all the NJ, ML and Bayesian trees. The NJ analysis was performed using the heuristic search, and a bootstrap procedure (Felsenstein, Reference Felsenstein1991) with 1000 replicates. The ML tree used the MP tree as the starting tree, and heuristic searches with as-is taxon addition and the TBR branch swapping algorithm with 1000 replicates. In the Bayesian procedure, 4 independent MCMC chains were simultaneously run for 1 000 000 replicates by sampling 1 tree per 100 replicates. The first 1000 trees sampled were discarded as part of a burn-in procedure, and the remaining 9000 sampling trees, whose log-likelihoods converged to stable values, were used to construct a 50% majority rule consensus tree. Consensus trees were drawn with Treeview 1.6.6 (Page, Reference Page2001). Alternative tree topologies were tested using Shimodaira-Hasegawa test (Shimodaira and Hasegawa, Reference Shimodaira and Hasegawa1999) also in PAUP*4.0b10.
RESULTS
Divergence of ITS-2 sequences
The variations (0–60·3%) at the level of sequence divergence were observed among species within the Diplozoinae examined herein (Table 2). High levels of interspecific similarities (>99%) were found for some congeneric species, i.e. among Paradiplozoon hemiculteri, P. parabramisi, P. parapeleci, P. opsariichthydis and P. jiangxiensis, and between Inustiatus inustiatus and I. aritichthysi (Table 2). The sequences for E. nipponicum were identical for specimens collected in China and those from the GenBank (Table 2). Species in Paradiplozoon in Europe and Diplozoon had 4·1–15·7% sequence divergence, and they together showed about 45·3–53·7% sequence divergence with Paradiplozoon in China. The Eudiplozoon showed about 26·9% sequence divergence with D. paradoxum, 24·9–27·5% with Paradiplozoon in Europe, if the view of Khotenovsky (Reference Khotenovsky1985) is accepted, about 28·8% with Sindiplozoon, 46·5–47·3% with Paradiplozoon in China, 33·4% with Inutiatus; and D. paradoxum showed 5·2–15·1% with Paradiplozoon in Europe, but 48·0–48·8% with Paradiplozoon in China, 20·5% and 37·3–37·8% with Sindiplozoon and Inustiatus, respectively. The Paradiplozoon in Europe had 20·0–23·7% sequence divergence with Sindiplozoon, 45·3–53·7% with Paradiplozoon in China, and 36·5–42·2% with Inustiatus. The Paradiplozoon in China had 58·5–60·3% sequence divergence with Inustiatus.
Pairwise distance (Kimura 2-parameter) matrix for the complete ITS2 sequences across all sequences from diplozoid species

Note: 1. The generic status was adopted from Khotenovsky (Reference Khotenovsky1985); Sind. represents Sindiplozoon.
2. Numbers represent percentage nucleotide divergence/difference. Numbers following species abbreviation are as those indicated in Table 1.
3. En=E. nipponicum; Dp=D. paradoxum; Db, D. bliccae; Pb, P. bliccae; Ps, P. sapae; Pn, P. nagibinae; Pp, P. pavlovskii; Dh, D. homoion; Ph, P. homoion; Pm, P. megan; Sc, S. ctenopharyngodoni; Po, P. opsariichthydis; Phe, P. hemiculteri; Ppb, P. parabramisi; Ppp, P. parapeleci; Pj, P. jiangxiensis; Ii and Ia, I. inustiatus and I. aristichthysi, respectively. Gaps/missing data: Pairwise deletion.
Phylogenetic analyses of ITS-2 sequences
Overall, the length of 29 full ITS-2 rDNA sequences ranged from 546 to 609 bp, and the G+C content from 45·4 to 48·0%. The complete alignment comprised 650 characters, of which 284 were variable and 251 parsimony informative (EMBL database ALIGN_000982).
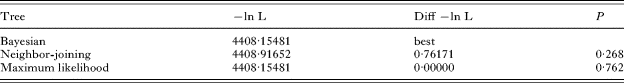
Phylogenetic analyses of the full ITS-2 sequences with N. hirame as an outgroup by NJ, ML and Bayesian methods produced essentially the same tree topology, with the Bayesian tree being the best (Table 3). The major difference among the 3 trees, although not significantly different, lies in the basal group: Eudiplozoon being the basal for ML tree, and the other 2 trees having Chinese Paradiplozoon as the basal.
Statistical comparison of topologies using Shimodaira-Hasegawa test
The NJ, ML and Bayesian trees strongly supported the presence of 4 groups of diplozoids, with the first being composed of species in the genus Diplozoon and species in Paradiplozoon from Europe only, the second of Eudiplozoon nipponicum, the third of species in Inustiatus, and the fourth of Paradiplozoon species from China (see BP values for NJ/ML/Bayesian trees in Figs 1, 2 and 3). Sindiplozoon ctenopharyngodoni and members of the group of Diplozoon sp. and European Paradiplozoon spp. form a large clade. The group of species in the Paradiplozoon from China forms the most basal clade to the Diplozoinae as revealed in NJ and Bayesian trees (Figs 1 and 3), and surprisingly they were separated in different clades from those in Paradiplozoon reported from Europe.
The neighbour-joining tree resulting from analysis of the complete ITS-2 rDNA sequences of diplozoid species using GTR+G model. The monogenean Neoheterobothrium hirame was used as outgroup.

The maximum-likelihood tree resulting from analysis of the complete ITS-2 rDNA sequences of diplozoid species using GTR+G model. The monogenean Neoheterobothrium hirame was used as outgroup.

Bayesian tree resulting from analysis of the complete ITS-2 rDNA sequences of diplozoid species using GTR+G model. The monogenean Neoheterobothrium hirame was used as outgroup.

DISCUSSION
The phylogenetic relationship among all 5 genera in the Diplozoinae was examined for the first time in the present study, with the inclusion of a total of 16 previously described species, i.e. 11 species of Paradiplozoon (2 of which were synonymized as Diplozoon species in several studies), 2 species of Inustiatus 1 species of Diplozoon, Eudiplozoon and Sindiplozoon respectively.
Molecular phylogenetic trees well supported the 2 clades representing Eudiplozoon and Inustiatus, respectively. The inclusion of the other 3 species reported in Sindiplozoon in China (Pan et al. Reference Pan, Zhang and Li1990) may then enable clarification of their phylogenetic relationship with other diplozoids. The fact that species in Paradiplozoon from Europe were clustered together with species in Diplozoon but separately with species in Paradiplozoon in China may suggest that Paradiplozoon spp. would be polyphyletic, if the taxonomic status of species in the Paradiplozoon in Europe was correct. The status of genera Diplozoon and Paradiplozoon needs to be revised, as suggested by previous authors (Matejusová et al. Reference Matejusová, Koubková and Cunningham2004). Also Le Brun et al. (Reference Le Brun, Renaud and Lambert1988) and Sicard et al. (Reference Sicard, Desmarais and Lambert2001) argued that D. bliccae, D. homoion, D. scardinii, and D. gracile should not be removed to Paradiplozoon. The present study supports the finding of previous authors and reports a significant divergence between European Paradiplozoon plus Diplozoon and Chinese Paradiplozoon. If the transfer of the above-mentioned diplozoids into genus Paradiplozoon by Khotenovsky (Reference Khotenovsky1981) is revised and rejected, 5 genera within the Diplozoinae would be sufficiently distinct on account of up to 20·0–60·3% overall pairwise ITS2 sequence divergence across genera.
It is, however, surprising that except for Diplozoon, all other genera in the Diplozoinae have been recorded in China, and the 2 genera, Sindiplozoon and Inustiatus may be considered specialists to Chinese fish as species in these 2 genera have only been found in China and in the Amur River which flows in China and also Russia (Wu et al. Reference Wu, Long and Wang2000).
Eudiplozoon nipponicum, originally described as D. nipponicum from Carassius carassius gibelio in Japan is generally found on the common carp C. carpio in Asia and Europe, as reported by others and in the present study (see Khotenovsky, Reference Khotenovsky1985; Wu et al. Reference Wu, Long and Wang2000). Lambert and Le Brun (Reference Lambert and Le Brun1988) suggested that the geographical distribution of hosts may play an important role in the occurrence and host-specificity of diplozoids. The carp is a native species in China, and is distributed throughout the country (Nie et al. Reference Nie, Yao, Gao, Wang and Zhang1999). It is suggested that E. nipponicum might have originated in the Far East and was subsequently transmitted to Europe with the transportation of its common carp host, being an introduced species in Europe. The unobserved divergences in ITS-2 sequences among 5 populations of E. nipponicum, i.e. 3 from China and 1 from the Czech Republic and France each, may imply that there is little or even no intraspecific variation for E. nipponicum during its colonization. This may also be interpreted as the short period of isolation and/or the existence of gene exchange as common carp has been transported frequently in Europe and also in China for either ornamental or aquaculture purposes (Hoole, Reference Hoole, Pike and Lewis1994; Nie et al. Reference Nie, Yao, Gao, Wang and Zhang1999).
If the Paradiplozoon represents Chinese species only, the Diplozoon appears to be a special group of diplozoids geographically restricted in Europe. In China and the Far East, there is the most diversified species composition of cyprinid fish in the World (Nelson, Reference Nelson1994) and this might reflect the diverse composition of diplozoids in the region (Khotenovsky, Reference Khotenovsky1985; Wu et al. Reference Wu, Long and Wang2000). It is likely that diplozoids might have evolved in this region and later on expanded into Europe. It appeared that Sindiplozoon is closely related to European Diplozoon; however their phylogenetic relationship to Eudiplozoon and Inustiatus is yet not fully solved. Further phylogenetic study should include more species collected in Asia and Europe and it would be of significant interest to investigate if diplozoids may have evolved with their cyprinid host fish.
Most diplozoid species are regarded as highly host specific, some being strictly host specific, with 1 parasite species associated with a single host species. In contrast, Diplozoon homoion has been recorded from more than 15 species of cyprinids (Khotenovsky, Reference Khotenovsky1985; Gelnar et al. Reference Gelnar, Šebelová, Dušek, Koubková, Jurajda and Zahrádková1997; Moravec et al. Reference Moravec, Gelnar, Ergens and Scholz1997). Sicard et al. (Reference Sicard, Desmarais and Lambert2001) speculated that unlike most other monogeneans which show strict host specificity, parasites in the Diplozoidae exhibit unusual heterogeneity in terms of host specificity, and considered that the host-specificity for parasites in the Diplozoidae may represent an intermediate situation between strict host specificity (1 host species) and wide host range. Nevertheless, host specificity should be interpreted cautiously in different species of diplozoids.
Diplozoid parasites also show low divergence in ITS-2 rDNA sequences at intraspecies level. Matejusová et al. (Reference Matejusová, Koubková and Cunningham2004) found no intra-specific variation for P. nagibinae, P. homoion and D. paradoxum from France and the Czech Republic, and detected identical sequences for different D. homoion populations. The low level of variations for species in China in Paradiplozoon observed in the present study ranged between 0 and 0·7% in ITS-2 sequence divergence across the geographical and xeno-populations, and this may raise the question on the identity of species in the Paradiplozoon in China. Similarly, the 2 species in the Inustiatus may also have such problems. These species and those in Paradiplozoon in Europe should thus be morphologically re-examined, and some other morphological characters should be identified for the classification.
The authors would like to thank many colleagues for their assistance in the collection of the parasites. The authors would like to thank sincerely three anonymous referees for their critical reviews on an earlier version, which have certainly improved the expression and ideas, and one referee has kindly corrected the English. This study was supported by a grant awarded to P. Nie from National Natural Science Foundation of China (Project No. 30025035) and a grant to P. Nie from the Chinese Academy of Sciences ([2005] 192).


