Introduction
The late Paleozoic witnessed one of the most important climatic events in Phanerozoic history known as the late Paleozoic ice age (LPIA; Montañez and Poulsen Reference Montañez and Poulsen2013). Although the classical view envisaged it as a protracted event encompassing one or few glaciations (Veevers and Powell Reference Veevers and Powell1987; Crowell Reference Crowell1999), the current understanding involves a complex climatic history of many different glaciations across Gondwana (Fielding et al. Reference Fielding, Frank and Isbell2008c; Henry et al. Reference Henry, Isbell and Limarino2008; Birgenheier et al. Reference Birgenheier, Fielding, Rygel, Frank and Roberts2009; Isbell et al. Reference Isbell, Henry, Gulbranson, Limarino, Fraiser, Koch, Ciccioli and Dineen2012; Montañez and Poulsen Reference Montañez and Poulsen2013).
Surprisingly, the current view of the LPIA dynamic climate contrasts with the proposed models about its impact on the marine biota. In this regard, authors have argued that the overall effect on the biota has been constant, beginning in the late Carboniferous and ending in the early Permian (Powell Reference Powell2005; Bonelli and Patzkowsky Reference Bonelli and Patzkowsky2011). The onset of major glaciation across Gondwana in the Serpukhovian (late Mississippian), caused a mass extinction of mostly paleotropical taxa with small latitudinal ranges (Powell Reference Powell2005, Reference Powell2007; McGhee et al. Reference McGhee, Sheehan, Bottjer and Droser2012). In turn, the intensity of the latitudinal diversity gradient decreased (Powell Reference Powell2007), and the global biogeographic structure caused a decline in origination and extinction rates leading to a sluggish macroevolutionary dynamic (Stanley and Powell Reference Stanley and Powell2003). Recently, some authors have analyzed the effect of these global dynamics on the ecological structure of paleotropical communities (Bonelli and Patzkowsky Reference Bonelli and Patzkowsky2008, Reference Bonelli and Patzkowsky2011; Heim Reference Heim2009; Badyrka et al. Reference Badyrka, Clapham and López2013). The results argue that regardless of important regional turnover coincident with the Serpukhovian mass extinction (Heim Reference Heim2009), during the LPIA paleotropical communities had low taxonomic turnover (Badyrka et al. Reference Badyrka, Clapham and López2013) and the hierarchical structure of the diversity, relative abundance distributions, and body-size distributions remained stable (Bonelli and Patzkowsky Reference Bonelli and Patzkowsky2008; Heim Reference Heim2009; Badyrka et al. Reference Badyrka, Clapham and López2013). These evidences suggested that the far-field biotic response to the waxing and waning of ice sheets was persistence rather than change (Bonelli and Patzkowsky Reference Bonelli and Patzkowsky2011).
Most of the evidence, however, comes from paleotropical regions, while regional-scale ecological analyses of ice-proximal basins are still scarce. Regional- to large-scale compositional and biogeographic studies of Gondwanan biotas (Kelley and Raymond Reference Kelley and Raymond1991; Shi and Waterhouse Reference Shi and Waterhouse2010; Sterren and Cisterna Reference Sterren and Cisterna2010; Clapham and James Reference Clapham and James2012; Dineen et al. Reference Dineen, Fraiser and Isbell2013; Waterhouse and Shi Reference Waterhouse and Shi2013) did suggest that major changes took place during the LPIA, indicating that regional ecological changes were possibly present. Such biogeographic and compositional changes, however, need not go hand in hand with regional ecological restructuring, and therefore, regional-scale analyses are needed to fully understand the nature of ecological changes facing the LPIA (Heim Reference Heim2009).
Because the Carboniferous successions from western Argentina record diverse marine faunas related to both major glacial intervals (Cisterna and Sterren Reference Cisterna and Sterren2008, Reference Cisterna and Sterren2010) and nonglacial intervals with temperate climates (Cisterna Reference Cisterna2010; Cisterna et al. Reference Cisterna, Sterren and Gutiérrez2011), they represent an ideal place to analyze the regional ecological changes related to the advance and retreat of glaciers during the LPIA. In this contribution I study the compositional turnover and change in the hierarchical structure and bathymetric gradient of diversity in western Argentina (Fig. 1) during the most extensive glaciation registered in the region (López Gamundí and Martínez Reference López Gamundí and Martínez2000; Henry et al. Reference Henry, Isbell and Limarino2008) and after its end (Limarino et al. Reference Limarino, Césari, Spalletti, Taboada, Isbell, Geuna and Gulbranson2014; Gulbranson et al. Reference Gulbranson, Montañez, Tabor and Limarino2015).
Location map of the study area depicting the basin paleogeography. Gray areas indicate positive topography. Sampling localities: RP, Río Blanco Anticlinal; QL, Quebrada Larga; H, Huaco area (Quebrada La Herradura and Quebrada La Delfina); DS, Quebrada del Salto; LC, La Capilla area (Las Cambachas and Las Juntas); ST, Sierra del Tontal. B, Barreal area (Barreal Anticlinal, Leoncito, Quebrada Majaditas, Cordón del Naranjo). CT, Cordillera del Tigre; AJ, Agua de Jagüel; SE, Quebrada Santa Elena.

Geological Setting
The late Paleozoic stratigraphy from western Argentina developed in a retroarc to arc-related basin (López Gamundí et al. Reference López Gamundí, Espejo, Conaghan and Powell1994; Astini et al. Reference Astini, Dávila, López Gamundí, Gómez, Collo, Ezpeleta, Martina and Ortiz2005). The Pennsylvanian–lower Permian stratigraphy is represented by the Paganzo Group and coeval units, which have recently been revised based on sequence stratigraphic (Limarino et al. Reference Limarino, Césari, Net, Marenssi, Gutiérrez and Tripaldi2002, Reference Limarino, Tripaldi, Marenssi and Fauqué2006; López Gamundí and Martínez Reference López Gamundí and Martínez2003; Desjardins et al. Reference Desjardins, Buatois, Limarino and Cisterna2009; Gulbranson et al. Reference Gulbranson, Montañez, Schmitz, Limarino, Isbell, Marenssi and Crowley2010), chronostratigraphic (Gulbranson et al. Reference Gulbranson, Montañez, Schmitz, Limarino, Isbell, Marenssi and Crowley2010; Césari et al. Reference Césari, Limarino and Gulbranson2011), biostratigraphic (Azcuy et al. Reference Azcuy, Beri, Bernardes-de-Oliveira, Carrizo, di Pasquo, Diaz Saravia, González, Iannuzzi, Lemos, Melo, Pagani, Rohn, Amenábar, Sabattini, Souza, Taboada and Vergel2007; Césari et al. Reference Césari, Limarino and Gulbranson2011; Cisterna et al. Reference Cisterna, Sterren and Gutiérrez2011), and paleogeographic (Geuna et al. Reference Geuna, Escosteguy and Limarino2010) aspects.
The Pennsylvanian starts with a major diamictite indicative of the late Serpukhovian–Bashkirian glaciation (Fig. 2), which is immediately followed by the postglacial transgression (Limarino et al. Reference Limarino, Tripaldi, Marenssi and Fauqué2006; López Gamundí Reference López Gamundí2010; Dineen et al. Reference Dineen, Fraiser and Isbell2013). This interval records the fauna from the Levipustula levis Taxon-range Zone (Cisterna and Sterren Reference Cisterna and Sterren2010) and coeval assemblages (Taboada Reference Taboada1997; Simanauskas and Cisterna Reference Simanauskas and Cisterna2001) that flourished in a diverse array of glacially influenced depositional environments. Stratigraphic and sedimentological analyses point out that the glaciomarine successions varied from ice proximal to ice distal, as wet-based tidewater glaciers advanced and retreated within fjords, while depositional environments ranged from deep (below storm wave base) to shallow (above storm wave base) marine (López Gamundí and Martínez Reference López Gamundí and Martínez2000; Henry et al. Reference Henry, Isbell, Limarino, McHenry and Fraiser2010; Alonso-Muruaga et al. Reference Alonso-Muruaga, Buatois and Limarino2013; Dineen et al. Reference Dineen, Fraiser and Isbell2013; Gulbranson et al. Reference Gulbranson, Isbell, Montañez, Limarino, Marenssi, Meyer and Hull2014). According to Limarino et al. (Reference Limarino, Tripaldi, Marenssi and Fauqué2006; see also Alonso Muruaga et al. 2013) the postglacial transgression is part of a third-order sequence (Fig. 2), while most of the glacial sediments belong to a previous sequence (Fig. 2).
Stratigraphic framework, sequence stratigraphy and chronostratigraphy of the studied region. Modified from Limarino et al. (Reference Limarino, Tripaldi, Marenssi and Fauqué2006), Césari et al. (Reference Césari, Limarino and Gulbranson2011), and Cisterna et al. (2010).
Overlying this glacially influenced interval, there is a period of continental to very shallow marine sedimentation that encompasses another third-order stratigraphic sequence (Fig. 2; Limarino et al. Reference Limarino, Tripaldi, Marenssi and Fauqué2006). Above this continental interval, another third-order stratigraphic sequence with an important transgression is present (Limarino et al. Reference Limarino, Tripaldi, Marenssi and Fauqué2006). Different marine intervals are present, interbedded with thin fluvial facies (Fig. 2), and have been related to a single Moscovian–Kasimovian transgression (Fig. 2; Limarino et al. Reference Limarino, Césari, Net, Marenssi, Gutiérrez and Tripaldi2002, Reference Limarino, Tripaldi, Marenssi and Fauqué2006; Desjardins et al. Reference Desjardins, Buatois, Limarino and Cisterna2009; Dineen et al. Reference Dineen, Fraiser and Isbell2013). Abundant evidence points toward a climatic amelioration during this interval (Limarino et al. Reference Limarino, Césari, Spalletti, Taboada, Isbell, Geuna and Gulbranson2014; Gulbranson et al. Reference Gulbranson, Montañez, Tabor and Limarino2015), with the presence of warm to temperate-water marine assemblages with a mixture of paleotropical and cool-water faunas (Cisterna Reference Cisterna2010; Taboada Reference Taboada2010; Cisterna et al. Reference Cisterna, Sterren and Niemeyer2014). This marine interval corresponds to the Tivertonia jachalensis–Streptorhynchus inaequiornatus Zone and related faunas (Sabattini et al. Reference Sabattini, Ottone and Azcuy1990; Cisterna Reference Cisterna2010; Cisterna et al. Reference Cisterna, Sterren and Gutiérrez2011).
Material and Methods
Data
For these analyses I compiled a presence-absence data set based on the literature. Only bed-level samples were used in the analyses, and literature resources related to each sample obtained are listed in the supplemental materials. Only brachiopod and bivalve genera were used in the analyses, with a total of 46 brachiopod genera and 42 bivalve genera. The final data set consists of 99 bed-level samples coming from 15 different localities (Fig. 1), totaling 88 genera and 481 occurrences (supplemental materials). Forty-four genera, summing 261 occurrences distributed in 48 samples come from the Bashkirian, while 51 samples with 60 genera and 245 occurrences are from the Moscovian–Kasimovian. All genera were classified in families, superfamilies, and orders. The Moscovian–Kasimovian part of the whole data set was already studied by Balseiro et al. (Reference Balseiro, Sterren and Cisterna2014).
Following published sedimentological analyses (e.g., López Gamundí Reference López Gamundí2001; Limarino et al. Reference Limarino, Césari, Net, Marenssi, Gutiérrez and Tripaldi2002, Reference Limarino, Isbell, Ciccioli and Taboada2013; Henry et al. Reference Henry, Isbell and Limarino2008, Reference Henry, Isbell, Limarino, McHenry and Fraiser2010; Alonso-Muruaga et al. Reference Alonso-Muruaga, Buatois and Limarino2013; Dineen et al. Reference Dineen, Fraiser and Isbell2013), all samples were classified in three depositional environments, namely shallow subtidal (above fair-weather wave base), deep subtidal (between fair-weather and storm wave bases), and offshore (below storm wave base). Although the number of samples is almost equal between intervals (48 Bashkirian and 51 Moscovian–Kasimovian samples), sampling coverage is clearly uneven between environments (Fig. 3).
Environmental sampling coverage of the studied intervals.
Sequence stratigraphic coverage is also relevant, because different system tracks could bias the nature of fossil beds due to differences in sedimentation rates (Scarponi and Kowalewski Reference Scarponi and Kowalewski2007). Samples from both intervals come from late-transgressive to early-highstand system tracks (Limarino et al. Reference Limarino, Tripaldi, Marenssi and Fauqué2006; Alonso Muruaga et al. 2013; Desjardins et al. Reference Desjardins, Buatois, Limarino and Cisterna2009), and therefore such biases would be minor.
Further taphonomic biases were tested previously by Balseiro et al. (Reference Balseiro, Sterren and Cisterna2014) for the Moscovian–Kasimovian interval, based on the taphonomic analysis carried out by Sterren (Reference Sterren2008) and the analytical framework put forward by Tomašových (Reference Tomašových2006). Balseiro et al. (Reference Balseiro, Sterren and Cisterna2014) showed that neither aragonite dissolution nor selectivity by storm reworking caused a significant bias in sample composition and diversity. Moreover, Balseiro et al. (Reference Balseiro, Sterren and Cisterna2014) also showed that there is no significant compositional turnover within the Moscovian–Kasimovian interval.
Methods
Temporal Turnover
For the analysis of taxonomic turnover, I used the analysis of similarity (ANOSIM; Clarke Reference Clarke1993). ANOSIM measures the difference between within-group mean rank distance and between-group mean rank distance (Legendre and Legendre Reference Legendre and Legendre2012). The analysis indicates this difference with a statistic called R that ranges from −1 to 1. R=1 if all within-group distances are lower than between-group distances, and R=0 if within and between-group distances are similar (Legendre and Legendre Reference Legendre and Legendre2012). R rarely has values lower than 0, because that would mean that between-group distances are lower than within-group distances (Legendre and Legendre Reference Legendre and Legendre2012). Using a simulation approach, Ivany et al. (Reference Ivany, Brett, Wall, Wall and Handley2009) showed that ANOSIM is a good proxy for taxonomic turnover. Warton et al. (Reference Warton, Wright and Wang2012) indicated that ANOSIM is sensitive to differences in multivariate dispersion. Therefore, I tested for homogeneity in multivariate dispersion before conducting the ANOSIM using a permutation test on a measurement of multivariate dispersion in a space defined by principal coordinates (Anderson Reference Anderson2006). To test for selectivity in the extirpation and immigration between brachiopods and bivalves, I used a chi-square test with Yates’s continuity correction.
I further analyzed the temporal turnover along the bathymetric gradient (Tomašových et al. Reference Tomašových, Dominici, Zuschin and Merle2014). I randomly subsampled without replacement eight samples from each environment in each interval and calculated the Bray-Curtis distance between Bashkirian and Moscovian–Kasimovian environments based on the eight pooled samples using both taxa occurrences and presence–absence. I chose eight samples for the resampling technique, because this is the minimum number of samples found in a given environment in a given time interval (Fig. 3). This subsampling was repeated 1000 times.
All analyses were performed in R (R Core Team 2015) with the vegan package (Oksanen et al. Reference Oksanen, Blanchet, Kindt, Legendre, Minchin, O’Hara, Simpson, Solymos, Stevens and Wagner2015). I used the anosim() function for the ANOSIM and betadisper() for the analysis of multivariate dispersion and chisq.test() for the chi-square test.
Ordination Analysis
For the study of biotic gradients, I used a nonmetric multidimensional scaling (NMDS; Legendre and Legendre Reference Legendre and Legendre2012). NMDS is a nonparametric technique that preserves the distance rank order between objects but not the actual distances between them (Legendre and Legendre Reference Legendre and Legendre2012). Furthermore, because it is a numerical approach, it makes no underlying assumption about the data.
Different analyses have shown that NMDS is as good as or better than other ordination techniques in recovering the underlying structure of the data (Minchin Reference Minchin1987; Bush and Brame Reference Bush and Brame2010). Recently, Alroy (Reference Alroy2015) proposed that principal coordinates analysis using a novel modification of the Forbes index was a best solution for paleoecological ordination. Using PCO and the Forbes index, or another common ordination technique such as detrended correspondence analysis, gave virtually identical results.
Bray-Curtis distance was used for the implementation of a two-dimension NMDS, using the metaMDS() function in the vegan package (Oksanen et al. Reference Oksanen, Blanchet, Kindt, Legendre, Minchin, O’Hara, Simpson, Solymos, Stevens and Wagner2015) for R (R Core Team 2015).
Diversity Analysis
I studied the structure of diversity using a hierarchical partition approach (Veech et al. Reference Veech, Summerville, Crist and Gering2002). Whittaker (Reference Whittaker1960, Reference Whittaker1972) was the first to propose that diversity could be partitioned in α, β, and γ components. He proposed that α diversity corresponded to local diversity (e.g., of a sample), while γ diversity corresponded to that of a region, with β diversity being the relationship between both scales. Initially, Whittaker (Reference Whittaker1960, Reference Whittaker1972) proposed a multiplicative relationship between local and regional scales expressed by the function,
 $$\gamma \,{\equals}\,\alpha \,{\times}\beta ^{{\times}} $$
where α is the average local diversity.
Later, several authors proposed that the relationship between different scales could be additive rather than multiplicative (MacArthur et al. Reference MacArthur, Recher and Cody1966; Levins Reference Levins1968; Veech et al. Reference Veech, Summerville, Crist and Gering2002). Lande (Reference Lande1996) formalized the additive partitioning of diversity, which is defined as,
 $$\gamma \,{\equals}\,\alpha {\plus}\beta ^{{\plus}} $$
The additive partition of diversity has the advantage of measuring all components (γ, α, β+) in the same units, making them easily comparable (Veech et al. Reference Veech, Summerville, Crist and Gering2002; Patzkowsky and Holland Reference Patzkowsky and Holland2012). Moreover, additive partitioning allows diversity to be partitioned along a hierarchy of scales (Veech et al. Reference Veech, Summerville, Crist and Gering2002; Patzkowsky and Holland Reference Patzkowsky and Holland2007, Reference Patzkowsky and Holland2012), allowing β diversity to be divide into different components.
However, it has been recently shown that additive partition is dependent on α (except for Shannon’s entropy [H']; see Jost Reference Jost2006, Reference Jost2007; Tuomisto Reference Tuomisto2010) and measures absolute compositional differences (Chao et al. Reference Chao, Chiu and Hsieh2012). The main problem related to this issue is that if α changes, then β+ will change regardless of whether the relative differences between samples remain stable. Moreover, if α changes, but β+ remains stable, it implies a change in the relative differences between samples rather than stability in β diversity (for further discussions, see Jost Reference Jost2006, Reference Jost2007; Tuomisto, Reference Tuomisto2010; Chao et al. Reference Chao, Chiu and Hsieh2012). To overcome this problem, I also used the relative turnover rate per community of Harrison et al. (Reference Harrison, Ross and Lawton1992), which can be derived from both multiplicative and additive β diversities and measures relative compositional differences and is not dependent on α (Chao et al. Reference Chao, Chiu and Hsieh2012). The rate is calculated as:
 $$Har\,{\equals}\,(\beta ^{{\asterisk}} -1)/(Nn-1)$$
where n is the total number of samples and β* is multiplicative β diversity. This rate measures the mean proportion of taxa that changes from one sample to another, and it ranges from 0, where there is no compositional change between samples, to 1, where all samples are different. I estimated additive β diversity in a sampling hierarchy using depositional environments. I calculated αs as mean sample diversity, αenv as mean environmental diversity, β+we as within-environment additive β diversity, and β+be as between-environment additive β diversity. Note that given this partition scheme, αenv=αs+β+we, while γ=αenv+β+be, which is the same as γ=αs+β+we+β+be. I also estimated turnover rates following this scheme.
Because sampling differed between environments and time intervals (Fig. 3), I standardized the number of samples using a resampling method. I subsampled eight samples per environment without replacement, for a total of 24 samples, and calculated additive diversity partition and turnover rates. This subsampling was repeated 1000 times to obtain mean values and confidence intervals based on the 2.5 and 97.5% percentiles.
Taxon Occupancy Curves
To understand the structure of taxon occurrences, I constructed ranked taxon occupancy curves (Fall and Olszewski Reference Fall and Olszewski2010; Jenkins Reference Jenkins2011). Occupancy has shown to be a very useful proxy for abundance both in recent (Holt et al. Reference Holt, Gaston and He2002) and fossil taxa (Ivany et al. Reference Ivany, Brett, Wall, Wall and Handley2009). Ranked taxon occupancy curves are analogous to rank order plots (also known as Whittaker plots or relative abundance curves) but differ in that the former plot occupancies and the latter relative abundance. In addition, ranked taxon occupancy curves are necessarily restricted to a set of samples or communities and therefore to regional or metacommunity scales. Hence, patterns in ranked occupancy curves help to identify underlying processes at such a scale (Fall and Olszewski Reference Fall and Olszewski2010; Jenkins Reference Jenkins2011).
Results
Temporal Turnover
Compositional differences at genus scale between Bashkirian and Moscovian–Kasimovian assemblages are observed in the NMDS, where samples from each interval are segregated in the ordination space (Fig. 4A). This pattern is confirmed by the ANOSIM, which shows significant turnover between Bashkirian and Moscovian–Kasimovian assemblages (R=0.289, p=2×10⁻⁴, homogeneity of dispersion p=0.662).
NMDS (non-metric multidimensional scaling) of the entire data set. A, Based on genera. B, Families. C, Superfamilies. D, Orders.
Compositional differences were also observed at higher taxonomic levels (Fig. 4B,C). Compositional differences at the familial (R=0.236, p<2×10⁻⁴, homogeneity of dispersion p=0.357), the superfamilial (R=0.194, p<2×10⁻⁴, homogeneity of dispersion p=0.662), and even the ordinal (R=0.101, p<2×10⁻⁴, homogeneity of dispersion p=0.077) levels were significant.
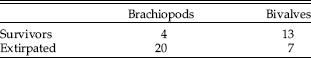
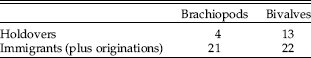
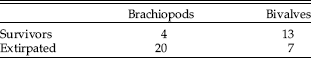
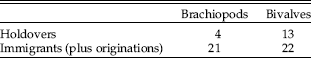
Further analyses show, however, that turnover is not uniform among brachiopods and bivalves, underscoring different turnover intensity between clades. A chi-square test of selectivity of extinction indicates that brachiopod genera suffer higher regional extinction than bivalves (Table 1, χ2=8.8072, df=1, p=0.003). Immigration (and/or origination), however, does not differ between clades, as both record similar numbers of new genera in the Moscovian–Kasimovian (Table 2, χ2=2.25, df=1, p=0.133).
Number of Bashkirian brachiopods and bivalves extirpated or surviving to the Moscovian–Kasimovian
Number of holdover or immigrants Moscovian–Kasimovian brachiopods and bivalves
Temporal turnover shows a clear trend along the bathymetric gradient. Figure 5B shows that the compositional differences between the Bashkirian and Moscovian–Kasimovian are clearly higher in the offshore than in shallower environments. The Bray-Curtis distance between intervals in all three environments is higher when dissimilarities are calculated using genera occupancies in each environment (Fig. 5B), but in this case, compositional differences in the offshore are even higher than in other environments (Fig. 5B).
A, NMDS of the entire data set showing the mean environmental position in the ordination space. B, Environment-scale temporal turnover measured as Bray-Curtis distance. Points are the means of 1000 subsamples, and error bars indicate 0.025 and 0.975 percentiles. ss, shallow subtidal; ds, deep subtidal; os, offshore.
Gradient Analysis
As mentioned above, the analysis of the whole data set shows that there is little overlap of Bashkirian and Moscovian–Kasimovian data sets in the ordination space (Fig. 4A). In addition, Bashkirian environmental centroids are more separated from one another than Moscovian–Kasimovian ones, suggesting that Bashkirian environments are a little more differentiated in the ordination space than Moscovian–Kasimovian environments (Fig. 5A). Interestingly, the Bashkirian shallow-subtidal centroid is located very close to the Moscovian–Kasimovian sample cluster, indicating that the highest compositional differences among intervals appear to be concentrated in the offshore and deep subtidal samples (Fig. 5A). This is confirmed by the analysis of compositional differences in each environment between intervals (Fig. 5B).
In the analysis of the Bashkirian data set, samples from all three environments overlap in the ordination space (Fig. 6A). The inability to cleanly segregate samples coming from different environments along the ordination space points to low compositional differentiation between environments (Fig. 6A). Nevertheless, there are some compositional differences that are confirmed by an ANOSIM (R=0.28, p=4×10⁻⁴). Samples coming from the deep subtidal tend to be placed toward higher values of axis 1, while offshore samples trend toward lower values (Fig. 6B). There is a large overlap between bivalves and brachiopods in the ordination space, and the nonsignificant segregation is confirmed by an ANOSIM (R=0.02, p=0.196).
A, B, NMDS of the Bashkirian data set. A, Ordination showing compositional differences between depositional environments. B, Ordination showing segregation of brachiopod and bivalves. C, D, NMDS of the Moscovian–Kasimovian data set. D, Ordination showing compositional differences between depositional environments. C, Ordination showing segregation of brachiopod and bivalves. Note that samples and taxa are plotted in the same ordination space.
Results of the ordination analysis of the Moscovian–Kasimovian data set show an interesting change in the structure of biotic gradients compared with the Bashkirian, namely, (1) there is a higher overlap of samples coming from different environments in the ordination space (Fig. 6C), indicating compositional similarities between environments (ANOSIM, R=−0.007, p=0.545); and more obviously (2) bivalves and brachiopods do segregate cleanly in the ordination space (Fig. 6D), underscoring the low co-occurrence of bivalves and brachiopods at sample scale (ANOSIM, R=0.18, p=2×10⁻⁴; homogeneity of dispersion, p=0.355; see also Balseiro et al. Reference Balseiro, Sterren and Cisterna2014).
Regional Diversity Partition
Gamma diversity shows a slight increase between the Bashkirian and Moscovian–Kasimovian (Fig. 7A). Interestingly, this small rise in γ diversity is not mirrored by αs diversity, which remains stable thought the studied intervals, but by αenv diversity. The driver of this pattern is, therefore, β diversity. The increase in αenv is clearly observed in Figure 7A. Although both β+we and β+be rise toward the Moscovian–Kasimovian, indicating an increase in absolute compositional differentiation within and between environments, Har we indicates that the main rise in relative compositional differentiation is concentrated within environments (Fig. 8A), while Har be remains stable, indicating a similar between-environment relative compositional differentiation (Fig. 8A).
Additive diversity partition of each time interval. From bottom to top (dark to light gray) partitions are αs, β+we, and β+be (see Methods for further explanation). Note that the total height of αs (dark gray bar) + β+we (medium-gray bar) equals αenv. Error bars are the 0.025 and 0.975 percentiles based on 1000 subsamples. A, Partition using all taxa. B, Bivalve partition. C, Brachiopod partition.
Relative turnover rate per community (Har) within environments and between environments in both intervals. Filled dots indicate mean, and error bars indicate the 0.025 and 0.975 percentiles based on 1000 subsamples. A, Har calculated using all taxa. B, Bivalve Har. C, Brachiopod Har.
In addition, β+we is much higher than αs both in the Bashkirian and the Moscovian–Kasimovian, indicating that αenv diversity is mostly explained by absolute compositional differences between samples.
When regional diversity patterns are dissected in brachiopods and bivalves, it is clear that these clades do not share a common pattern. Brachiopods show a rather stable pattern with a slight decrease in γ diversity toward the Moscovian–Kasimovian that is mirrored by αs but not by αenv diversity (Fig. 7C); consequently, Har we rises, indicating that within-environment community differentiation increased in the Moscovian–Kasimovian (Fig. 8C). Finally, the stability between Bashkirian and Moscovian–Kasimovian environmental diversity (αenv) causes both β+be and Har be to decrease (Figs. 6C and 7C), indicating that environments became compositionally more similar toward the Moscovian–Kasimovian.
On the other hand, bivalves show an increase in all αs, αenv, and γ diversities (Fig. 7B). This increment is also mirrored by a rise in both β+we and Har we (Figs. 6B and 7B), underscoring that similarly to brachiopods, bivalves demonstrated an increase in within-environment community differentiation in the Moscovian–Kasimovian. Bivalves’ β+be also rose toward the Moscovian–Kasimovian, but Har be remained stable (Figs. 6B and 7B). This latter incongruity is caused by the joint rise in αenv and γ and indicates that proportional compositional difference between environments remained stable, although the absolute number of genera that differed increased.
Bathymetric Diversity Gradient
The regional pattern can also be dissected along the environmental gradient, as shown in Figure 9. There is an interesting change in the structure of the bathymetric diversity gradient between the Bashkirian and Moscovian–Kasimovian, and brachiopods and bivalves share rather similar diversity gradients in each interval. In the Bashkirian, the environmental γ-diversity gradient is clearly hump shaped, with the deep subtidal being the most diverse environment and the shallow subtidal being slightly more diverse than the offshore (Fig. 9A). The latter is more clearly observed in bivalves than brachiopods (Fig. 9C,E). In contrast to γ diversity, αs is similar for the shallow and deep subtidal but decreases toward the offshore, although this is not significant given the confidence interval (Fig. 9A). Regarding β diversity, the regional pattern indicates that the deep subtidal has the highest β+ and Har along the environmental gradient (Figs. 9A and 10A). Although bivalves also record a clear difference in β+ and Har between the deep subtidal and the other two environments (Figs. 9C and 10C), brachiopods only show this pattern for β+, while Har for the offshore almost equals that of the deep subtidal (Figs. 9E and 10E). As in previous cases, this difference indicates that although absolute compositional differences were higher in the deep subtidal brachiopod communities, relative differences were similar in both environments.
Additive diversity partition along the bathymetric gradient in each interval. Partitions are αs (dark gray) and β+we (light gray); see Methods for further explanation. A, Bashkirian partition using all taxa. B, Moscovian–Kasimovian partition using all taxa. C, Bivalve Bashkirian partition. D, Bivalve Moscovian–Kasimovian partition. E, Brachiopod Bashkirian partition. F, Brachiopod Moscovian–Kasimovian partition.
Relative turnover rate per community (Har) within environments along the bathymetric gradient in both intervals. A, Bashkirian Har values using all taxa. B, Moscovian–Kasimovian Har values using all taxa. C, Bivalve Bashkirian Har values. D, Bivalve Moscovian–Kasimovian Har values. E, Brachiopod Bashkirian Har values. F, Brachiopod Moscovian–Kasimovian Har values.
During the Moscovian–Kasimovian, on the other hand, the bathymetric diversity gradient had a linear shape, reaching its maximum toward the deepest environments (Fig. 9B), although I should note that the deep subtidal shows large variability in the subsampled γ diversity, reaching higher maximum diversity than the offshore. Regardless of this last issue, it is worth noting that the offshore is definitely more diverse that the shallow subtidal. The higher offshore γ diversity is clearly observable in bivalves (Fig. 9D), while in brachiopods shallow-subtidal γ diversity is not so evidently lower than offshore γ diversity (Fig. 9F).
The trend in αs within each environment is also linear with higher values in the offshore (Fig. 9B), and both bivalves and brachiopods mirror this pattern (Fig. 9D,F). Interestingly, while β+ also follows a linear gradient with higher values in the offshore (Fig. 9), Har shows a humped trend with the highest values in the deep subtidal (Fig. 10B). Bivalves and brachiopods share the pattern in β+ (Fig. 9D,F) but differ in Har. Brachiopods have similar Har values in the shallow subtidal and deep subtidal, while the offshore records the lowest values (Fig. 10F). Bivalves, on the other hand, have a humped pattern with higher values of Har in the deep subtidal (Fig. 10B). This discrepancy between the environmental gradient of β+ and Har again underscores the differences between absolute and relative compositional differences along the bathymetric gradient and among clades.
Besides the pattern in environmental diversity within each interval, there is an interesting shift in the actual values from the Bashkirian toward the Moscovian–Kasimovian. While αs decreases in the Moscovian, both in the shallow subtidal and deep subtidal, in the offshore αs is clearly higher during this interval. Regarding environmental γ diversity, the shallow subtidal again seems to be more diverse during the Bashkirian; the deep subtidal, however, shows virtually no difference between intervals. The offshore, on the other hand, is definitely more diverse during the Moscovian–Kasimovian, almost doubling in richness the Bashkirian deepest environment.
Brachiopods have slightly higher shallow- and deep-subtidal γ diversity during the Bashkirian, but much higher offshore diversity during the Moscovian–Kasimovian. Bivalves, meanwhile, have almost identical shallow-subtidal diversity in both intervals and show a small rise in deep subtidal diversity during the Moscovian–Kasimovian. Bivalves, again, record an increase in offshore γ diversity, but this time the shift is almost a threefold rise in the Moscovian–Kasimovian.
Regarding β diversity, there is a common pattern for both brachiopods and bivalves, with a virtual stability in shallow-subtidal and deep-subtidal β+ diversity and a rise in offshore β+. The increase in offshore β+ differs in magnitude between clades, being much higher in bivalves, again having a threefold increment. Temporal trends in Har, however, indicate a different pattern for relative compositional differentiation within environments. While brachiopods show a rise in shallow- and deep-subtidal Har and stability in offshore Har, bivalves record a small rise in all three environments. The regional pattern is, therefore, a rather clear rise in shallow- and deep-subtidal Har, and a smaller rise in offshore Har.
All in all, environmental diversity patterns underscore that although all three environments show differences between the Bashkirian and Moscovian–Kasimovian, the most important changes are recorded in the offshore. Here, there was an important rise in inventory diversities that made the environmental diversity gradient shift from a humped pattern in the Bashkirian to a linear pattern in the Moscovian–Kasimovian. Interestingly, shallow- and deep-subtidal settings recorded the most important shifts in within-environment relative compositional differentiation (Har), while the offshore exhibited the highest absolute differentiation (β+).
Taxa Occupancy Patterns
To further understand which taxa were involved in the diversity changes, I analyzed taxon occupancy curves for both clades together and separately during the Bashkirian and Moscovian–Kasimovian. The occupancy curves for all taxa are very similar between intervals (Fig. 11A), which indicates that there is no shift in the commonness of taxa and highlights that the increase in γ diversity is mostly caused by the gain of rare taxa in the Moscovian–Kasimovian. Interestingly, brachiopods and bivalves do not share a similar pattern. While brachiopods show a decrease in the occupancy of intermediately frequent genera toward the Moscovian–Kasimovian (Fig. 11C), bivalves have the opposite trend, with a rise in occupancies of intermediate genera (Fig. 11B). The fact that both clades have opposite patterns causes the regional picture to remain stable.
Ranked taxon occupancy curves. Shaded areas are 95% confidence intervals based on 1000 bootstraps. A, Curves for all taxa. B, Bivalve curve, C, Brachiopod curve.
Further analyses shows that despite the regional stability in the occupancy distribution, there are changes in each taxon occupancy between the Bashkirian and the Moscovian–Kasimovian. Occupancy changes of surviving genera are small and positively correlated between intervals (Kendal’s correlation τ=0.401, p=0.033). Shifts in occupancies, however, are present at higher taxonomic levels. Both families (Kendal’s correlation τ=0.2, p=0.856) and superfamilies (Kendal’s correlation τ=0.191, p=0.124) occupancies are not significantly correlated between intervals. The number of genera per family and superfamily also lack correlation between intervals (Kendal’s correlation τ=−0.18 and −0.022, p=0.155 and 0.875, respectively) indicating that not only occupancies changed but also richness within (super)families.
Furthermore, brachiopod and bivalve occurrences at sample scale reinforce the change in segregation patterns observed in the ordination analyses between Bashkirian and Moscovian–Kasimovian assemblages. Figure 12 shows that the distribution of the proportion of brachiopod occurrences is bimodal during the Moscovian–Kasimovian. Many samples have a proportion of brachiopod occurrences higher than 0.9, while a second large group of samples have a proportion lower than 0.1. There are a much lower number of samples with proportional occurrences of brachiopods ranging from 0.3 to 0.7. This pattern underscores that most samples were either exclusively dominated by brachiopods or bivalves. During the Bashkirian, on the other hand, many samples had intermediate (0.3–0.7) values of proportional occurrences of brachiopods, and there is no evidence of a bimodal distribution. This pattern suggests that brachiopods and bivalves tend to co-occur at sample scale during the Bashkirian. There are many samples with proportional occurrences of brachiopods higher than 0.9, but this is probably caused by higher occupancies of brachiopods compared with bivalves during this interval.
Discussion
Stability or Change?
Different authors have analyzed the effect of the LPIA in the ecological structure of paleotropical ecosystems (Bonelli and Patzkowsky Reference Bonelli and Patzkowsky2008, Reference Bonelli and Patzkowsky2011; Powell Reference Powell2008; Heim Reference Heim2009; Badyrka et al. Reference Badyrka, Clapham and López2013). The current understanding of the marine biotic consequences of the LPIA is a constant protracted response of the benthic communities, starting with a mass extinction coinciding with the major development of the ice caps at the Serpukhovian (Raymond et al. Reference Raymond, Kelley and Lutken1990; Powell Reference Powell2008; McGhee et al. Reference McGhee, Sheehan, Bottjer and Droser2012). Despite important regional taxonomic turnover registered at the onset of the major glaciation (Powell Reference Powell2008; Heim Reference Heim2009), evidence indicates that during the LPIA: (1) regional biotic gradients were short and recurred with high fidelity between depositional sequences (Bonelli and Patzkowsky Reference Bonelli and Patzkowsky2008), (2) diversity and relative abundance distributions remained somewhat stable both at the beginning and throughout the LPIA (Bonelli and Patzkowsky Reference Bonelli and Patzkowsky2008, Reference Bonelli and Patzkowsky2011; Heim Reference Heim2009; Badyrka et al. Reference Badyrka, Clapham and López2013, but see Powell Reference Powell2008), and (3) faunal turnover was low (Olszewski and Patzkowsky Reference Olszewski and Patzkowsky2001a; Heim Reference Heim2009; Bonelli and Patzkowsky Reference Bonelli and Patzkowsky2011; Badyrka et al. Reference Badyrka, Clapham and López2013). These patterns led Bonelli and Patzkowsky (Reference Bonelli and Patzkowsky2011) to suggest that the biotic response to the late Paleozoic icehouse was taxonomic and ecological persistence.
In this scenario, one could expect similar patterns at higher latitudes or even greater stability and lower turnover, given that the extinction at beginning of the LPIA was concentrated in paleotropical regions (Powell Reference Powell2005, Reference Powell2007). The present results, however, point to a very different pattern, as glacially influenced regions record significant turnover even at intermediate latitudes (Table 1). In any case, new (immigrants) and extirpated genera are mainly range-through taxa (Cisterna Reference Cisterna2010), indicating that although important, turnover was only a regional-scale process.
It has to be stressed, however, that there are substantial differences in the temporal resolution between this contribution and some paleotropical studies and even among paleotropical studies (Olszewski and Patzkowsky Reference Olszewski and Patzkowsky2001a,Reference Olszewski and Patzkowskyb; Powell Reference Powell2008; Heim Reference Heim2009; Bonelli and Patzkowsky Reference Bonelli and Patzkowsky2011; Badyrka et al. Reference Badyrka, Clapham and López2013). In particular, the current study differs in temporal scale with Bonelli and Patzkowsky (Reference Bonelli and Patzkowsky2011), which spans 11 intervals within 3 Myr, and Olszewski and Patzkowsky (Reference Olszewski and Patzkowsky2001a,Reference Olszewski and Patzkowskyb), which spans 31 intervals within 12.5 Myr. Such variability in temporal resolution could be the reason for the observed differences in turnover between regions. However, other paleotropical studies do encompass larger time intervals. For example, Heim (Reference Heim2009) compared Chesterian (Mississippian) with Morrowan (Pennsylvanian) assemblages spanning ~21 Myr; while Badyrka et al. (Reference Badyrka, Clapham and López2013) studied three intervals Moscovian (Pennsylvanian) and Asselian and Sakmarian (lower Permian) encompassing ~21 Myr. Given the similarities in temporal resolution between this contribution and Heim (Reference Heim2009) and Badyrka et al. Reference Badyrka, Clapham and López2013), differences between paleotropical and ice-proximal regions are difficult to explain based on temporal resolution alone.
The observed compositional turnover, however, should not necessarily generate large ecological changes (McGhee Reference McGhee1981; Droser et al. Reference Droser, Bottjer, Sheehan and McGhee2000; Christie et al. Reference Christie, Holland and Bush2013), since it is possible that newly arrived taxa were phylogenetically, and hence ecologically (Burns and Strauss Reference Burns and Strauss2011), related to those extirpated. This seems not to be the case in western Argentina. On the one hand, while extirpation was much more intense in brachiopods than bivalves, immigration was similar in both clades, leading to a change in the brachiopods:bivalves ratio and causing a major change in the taxonomic structure of the metacommunities. During the Bashkirian the brachiopods:bivalves ratio was 20:17 for genera and 131:85 for occurrences, while toward the Moscovian–Kasimovian these ratios decrease to 19:26 for genera and 118:127 for occurrences, which means an important reduction in the number of brachiopod genera and occurrences relative to bivalves. Although the taxon occupancy curve remains stable, each clade presents an opposite response, namely an increase in the occupancies of intermediate taxa in bivalves and a decline in brachiopods.
On the other hand, although—as expected—environmental change struck with varying degrees at different taxonomic hierarchies, consequences are visible even at the suprafamilial level, causing changes in generic occupancies and identity of diverse and frequent (i.e., high-occupancy) families (Sterren and Cisterna Reference Sterren and Cisterna2010). Diversity and occupancy rank order of families is uncorrelated between intervals, underscoring that the most important families in Moscovian–Kasimovian communities were rare or directly absent during the Bashkirian.
Interestingly, Clapham and James (Reference Clapham and James2008) also found relevant turnover during the LPIA in glaciated eastern Gondwana (lower–middle Permian, Australia) across different glacial–nonglacial transitions (Fielding et al. Reference Fielding, Frank, Birgenheier, Rygel, Jones and Roberts2008b; Birgenheier et al. Reference Birgenheier, Fielding, Rygel, Frank and Roberts2009). Heim (Reference Heim2009) also described a pattern of turnover and ecological change similar to the results presented here but at low-latitude Laurasia, namely: (1) high regional turnover of mostly global range-through taxa, and (2) stability in relative abundance distribution but change in the identity of abundant and rare taxa. Heim’s (Reference Heim2009) findings, however, were related to the mass extinction at the beginning of the LPIA. Badyrka et al. (Reference Badyrka, Clapham and López2013), on the other hand, did not find large compositional changes during the LPIA in low-latitude western Gondwana (Pennsylvanian–lower Permian, Bolivia), although their studied interval did span several glaciations elsewhere in Gondwana (López Gamundí Reference López Gamundí1997; Fielding et al. Reference Fielding, Frank, Birgenheier, Rygel, Jones and Roberts2008a; Isbell et al. Reference Isbell, Fraiser and Henry2008; Montañez and Poulsen Reference Montañez and Poulsen2013). Hence, paleoequatorial communities might have suffered little during ice-cap advance and retreat at high latitudes (Bonelli and Patzkowsky Reference Bonelli and Patzkowsky2011; Badyrka et al. Reference Badyrka, Clapham and López2013), while in glaciated regions those passages caused significant changes in the biota. These differences could be explained if, while high-latitude oceans had important temperature fluctuations, the surface temperature of tropical oceans remained stable along the LPIA with, albeit, a reduction of the low-latitude warm belt (Angiolini et al. Reference Angiolini, Jadoul, Leng, Stephenson, Rushton, Chenery and Crippa2009; Montañez and Poulsen Reference Montañez and Poulsen2013). Another possibility could be that high-latitude faunas were not culled of glacial-sensitive taxa such as the tropical fauna by the Serpukhovian mass extinction and therefore did not witness a change in their turnover dynamics through the LPIA. Unfortunately, more analyses and comparisons are needed to test this last possibility.
Where Did Change Concentrate?
The slight increase in β diversity, both in absolute (β+) and relative (Har) values, can be interpreted as an increase in patchiness or in dispersal limitation during the Moscovian–Kasimovian. Such a change occurred strictly among local communities, because β diversity between environments did not change in either absolute or relative values. As dispersal limitation should have also affected the between-environment differentiation and modified the occupancy distribution (Fall and Olszewski Reference Fall and Olszewski2010), the results support a change in patchiness rather than in dispersal limitation. Heim (Reference Heim2009) also found lower between-local communities differentiation after the onset of the major mid-Carboniferous glaciations in paleotropical Laurussia, suggesting that the loss of local patchiness was a common environmental response at the face of glacial advance at both high- and low-latitude regions.
Nevertheless, the consequences of environmental change are much more complicated. The environmental diversity gradient changed dramatically from a humped gradient toward a linear gradient as the glaciers declined in western Argentina. As mentioned before, shallow- and deep-subtidal γ diversity remained rather stable between intervals, while offshore diversity rose. The fact that the Har environmental gradient remains humped in both intervals, despite the environmental changes in inventory diversities, sheds light on the underlying dynamics of the ecological change caused by the waning of glaciers. The increase in offshore γ diversity during the Moscovian–Kasimovian was most probably not caused by an increase in within-environment variability (i.e., patchiness), because offshore Har remained stable, indicating that relative differences among offshore samples did not change between intervals. The rise in offshore γ diversity was therefore driven almost exclusively by the gain in offshore αs. An increase in αs diversity could be caused by different factors, such as a change in a limiting factor like salinity or oxygen (Shi et al. Reference Shi, Zhang, Shen and He2015). Independent evidence from trace fossils suggests that intervals differed in salinity, caused by higher meltwater discharge during the Bashkirian, but not in oxygenation (Desjardins et al. Reference Desjardins, Buatois, Mángano and Limarino2010). Such a change in salinity should have triggered a rise in shallow-subtidal αs rather than in offshore αs, and therefore does not seem to have controlled changes in the bathymetric diversity gradient. The rise in offshore αs could have also been driven by an increase in local resource availability (Kaspari et al. Reference Kaspari, O’Donnell and Kercher2000; Hurlbert Reference Hurlbert2004) or a more efficient resource partitioning (i.e., higher evenness) (Tokeshi Reference Tokeshi1999). Unfortunately, the lack of relative abundance data limits a proper analysis of the relative importance of these two last possibilities. Nevertheless, the fact that bivalves, which have a higher energetic demand compared with brachiopods (Payne et al. Reference Payne, Heim, Knope and McClain2014), showed a more pronounced diversity and occupancy rise suggests that resource availability (i.e., food) could have had more relevance. Moreover, αs almost doubled from the Bashkirian (αs=4) to the Moscovian (αs=7.16), and such an increment is difficult to explain by a rise in evenness alone (i.e., higher resource partitioning). Therefore, although both variables were possibly acting together, an increase in resources might have had more relevance in the observed rise of offshore αs.
Because a reduction in food availability toward shallow environments seems unlikely, the decline in αs toward the shallow and deep subtidal is most probably related to the humped relationship between diversity and productivity (Rosenzweig Reference Rosenzweig1995) and therefore to an even higher increase in resource availability in these environments. Despite this decrease in αs, shallow- and deep-subtidal γ diversity remained stable due to the rise in Har, indicating a parallel rise in patchiness and resource availability.
It is extremely interesting that both brachiopods and bivalves show a similar change in the shape of the gradient, indicating that the factor that generated such a shift affected both clades alike. However, because the magnitude of some changes differ between clades it is also remarkable that there were idiosyncratic responses. Bivalves show a more pronounced rise in offshore αs diversity (Fig. 8C,D), while brachiopods show a more pronounced decrease in shallow- and deep-subtidal αs (Fig. 9E,F). In addition, brachiopods also seem to have been more affected by the increase in patchiness in the shallow and deep subtidal, as evidenced by the rise in Har (Fig. 9E,F), suggesting that they were probably more affected by subtle environmental differences.
Both the environmental turnover gradient (Fig. 5B) and the changes in the diversity gradient (Fig. 9A,B) suggest that the largest changes occurred toward the offshore. Interestingly, Clapham and James (Reference Clapham and James2008) also found that the compositional change started in deep environments during the fade of the LPIA in high latitudes of eastern Gondwana. This is surprising, because one might expect major changes to occur in shallow environments, which face the harshest conditions during glacial intervals and suffer the greatest changes in postglacial intervals, either through meltwater discharge (Buatois et al. Reference Buatois, Netto and Mángano2010, Reference Buatois, Netto, Gabriela Mángano and Carmona2013; Alonso-Muruaga et al. Reference Alonso-Muruaga, Buatois and Limarino2013) or temperature fluctuations. Indeed, extinction at the beginning of the LPIA seems to have preferentially targeted shallow taxa in the Appalachian Basin (Powell Reference Powell2008). Moreover, different evidence suggests that at macroevolutionary scales, shallow environments record major compositional changes compared with deep environments (Tomašových et al. Reference Tomašových, Dominici, Zuschin and Merle2014). These results, therefore, highlight that high-latitude communities responded very differently to the fade of major glaciations than did low-latitude communities to their onset, and probably even nonglacial communities in general.
Changes in Bivalve–Brachiopod Coexistence
The fact that analyzing both clades together shows certain stability in the diversity structure could suggest that the metacommunities responded to neutral dynamics (Heim Reference Heim2009), wherein all taxa were nearly ecological equivalents and compositional changes were caused mainly by stochastic processes such as ecological drift and dispersal (Hubbell Reference Hubbell2001, Reference Hubbell2006). Then, the differential extirpation and migration of brachiopods and bivalves were casual processes that did not affect the regional ecological structure. Analyzing regional patterns is, however, only one side of the coin, and the analyses of local coexistence indicate a very different pattern of nonneutral dynamics (Balseiro et al. Reference Balseiro, Sterren and Cisterna2014). While brachiopods and bivalves coexisted at the local scale during the Bashkirian, coexistence did not occur in Moscovian–Kasimovian communities (Fig. 12; Balseiro et al. Reference Balseiro, Sterren and Cisterna2014).
Histograms showing the proportion of brachiopod genera per sample. Note the different distributions between the Bashkirian (unimodal) and Moscovian–Kasimovian (bimodal).
Lack of coexistence at the local scale could be caused by different factors. Balseiro et al. (Reference Balseiro, Sterren and Cisterna2014) already analyzed whether this pattern was caused by taphonomic biases such as aragonite dissolution or storm reworking and showed that neither possibility could explain it. One explanation could be that higher within-environment variability (i.e., patchiness) during the Moscovian–Kasimovian caused an environmental checkerboard that segregated brachiopods and bivalves at sample but not larger scales (i.e., environmental). However, in such a scenario one should expect to find some sort of segregation during the Bashkirian, because it is difficult to believe that Moscovian–Kasimovian within-environment variability exerted stronger segregation than Bashkirian between-environment variability. In other words, it could be possible that during one interval brachiopods and bivalves were segregated at the environmental scale and later such segregation was only visible at the sample but not at a larger scale due to lower between-environment but higher within-environment variability (i.e., an environmental checkerboard). However, western Argentina did not witness a shift in scale at which brachiopods and bivalves segregate. A related possibility to explain changes in coexistence is a difference in preserved environmental variability caused by a time-averaging bias. If time averaging was higher during the Bashkirian, then brachiopods and bivalves would appear to coexist at the sample scale even though they were actually segregated, because time averaging transfers diversity from β to alpha levels (Tomašových and Kidwell Reference Tomašových and Kidwell2009). However, time averaging should have been lower, not higher, during glacial intervals (i.e., Bashkirian) due to higher sedimentation rates caused by glacial erosion (Montgomery Reference Montgomery2002). Moreover, if differences in coexistence were caused only by higher time averaging during the Bashkirian, then both brachiopods and bivalves should share the same pattern of change in α and β diversity from the Bashkirian to the Moscovian–Kasimovian (Tomašových and Kidwell Reference Tomašových and Kidwell2009), but that is not the case in western Argentina (Fig. 7).
Previously, Balseiro et al. (Reference Balseiro, Sterren and Cisterna2014) suggested that low or absent bivalve–brachiopod coexistence during the Moscovian–Kasimovian was not caused by taphonomic biases or by geographic, temporal, or environmental factors. Moreover, as low coexistence was also not explained by neutral dynamics, they showed that it was probably related to competition (Balseiro et al. Reference Balseiro, Sterren and Cisterna2014). This implies that brachiopods and bivalves were able to coexist during the Bashkirian but were later segregated by competitive interaction. Unfortunately, it is very difficult to assert why competition became stronger during the Moscovian–Kasimovian. The waxing and waning of glaciers during the LPIA, therefore, not only caused major taxonomic turnover and modified the shape of the bathymetric diversity gradient but also caused major changes in community assembly dynamics by strengthening the effect of competition on the composition of local communities. This change indicates a shift from a system in which community assembly is not regulated by interactions to a system in which local dynamics are dominated by competition (DiMichele et al. Reference DiMichele, Behrensmeyer, Olszewski, Labandeira, Pandolfi, Wing and Bobe2004). Moreover, such a shift indicates that the dynamics underlying local community assembly can be modified at the temporal scale used in this study. The fact that much research has shown that communities in the fossil record respond to either dynamic (DiMichele et al. Reference DiMichele, Pfefferkorn and Gastaldo2001; Olszewski and Patzkowsky Reference Olszewski and Patzkowsky2001b; Patzkowsky and Holland Reference Patzkowsky and Holland2003; DiMichele et al. Reference DiMichele, Behrensmeyer, Olszewski, Labandeira, Pandolfi, Wing and Bobe2004; Ivany et al. Reference Ivany, Brett, Wall, Wall and Handley2009; Balseiro and Waisfeld Reference Balseiro and Waisfeld2013) could indicate that such shifts are more common than previously thought. More research, however, needs to be conducted to determine the actual temporal and geographical patterns of these possible changes in community assembly dynamics.
Conclusions
Although the relationship is not perfect, it is generally assumed that the higher the turnover rates, the higher the ecological consequences (McGhee et al. Reference McGhee, Clapham, Sheehan, Bottjer and Droser2013). Indeed, many studies have analyzed how mass extinctions caused significant ecological changes within biota (e.g., Tomašových and Siblík Reference Tomašových and Siblík2007; Heim Reference Heim2009; Danise et al. Reference Danise, Twitchett, Little and Clémence2013; McGhee et al. Reference McGhee, Clapham, Sheehan, Bottjer and Droser2013; Aberhan and Kiessling Reference Aberhan and Kiessling2015), while less effort has been focused on intervals of background extinction rates (e.g., Tang and Bottjer Reference Tang and Bottjer1996; Olszewski and Patzkowsky Reference Olszewski and Patzkowsky2001b; Patzkowsky and Holland Reference Patzkowsky and Holland2007; Fall and Olszewski Reference Fall and Olszewski2010). In fact, because the LPIA was an interval of sluggish macroevolutionary dynamics dominated by large-range taxa, Bonelli and Patzkowsky (Reference Bonelli and Patzkowsky2011) suggested that the LPIA was an interval of ecological persistence. However, results from western Argentina underscore that regional-scale ecological changes during the LPIA in high-latitude regions included: (1) high extirpation of brachiopods causing significant changes in the structure of the metacommunities, (2) modifications of the bivalve hierarchical diversity structure, (3) remodeling of the bathymetric diversity gradient, and (4) changes in the bivalve–brachiopod local-scale coexistence indicating shifts in communities assembly dynamics. Such ecological modifications were of similar magnitude to those observed at the Serpukhovian mass extinction in paleotropical basins (Bonelli and Patzkowsky Reference Bonelli and Patzkowsky2008, Reference Bonelli and Patzkowsky2011; Heim Reference Heim2009), suggesting that the waxing and waning of glaciers was able to cause regional taxonomic turnover and medium-scale ecological changes even during intervals of relative macroevolutionary quiescence (Stanley and Powell Reference Stanley and Powell2003; Powell Reference Powell2005; Stanley Reference Stanley2007).
Acknowledgments
The author would like to thank A. F. Sterren (CICTERRA, CONICET and Universidad Nacional de Córdoba) and G. A. Cisterna (CONICET and Universidad Nacional de La Rioja) for the invaluable help provided in the construction of the database and for sharing their knowledge about systematic, stratigraphic, paleoenvironmental, and biostratigraphic issues. Matthew Powell (Juniata College), Mark Patzkowsky (Pennsylvania State University), and an anonymous reviewer are thanked for their thoughtful suggestions, which significantly improved this contribution. The Consejo Nacional de Investigaciones Científicas y Técnicas (CONICET) and the Universidad Nacional de Córdoba provided support and facilities used in this investigation. Financial support was provided by the ANPyT (Agencia Nacional de Promoción Científica y Tecnológica)-FONCYT (Grant PICT-2014-3058).
Supplementary Material
Supplemental material deposited at Dryad: doi:10.5061/dryad.04gj1