Introduction
The evolution of herbicide resistance in weeds has a significant impact on the sustainability of food production across the globe (Beckie and Tardif Reference Beckie and Tardif2012), and the number of herbicide-resistant weed species continues to increase (Heap Reference Heap2018). Multiple herbicide resistance has been confirmed in many weed species globally (Keshtkar et al. Reference Keshtkar, Mathiassen, Moss and Kudsk2015; Owen et al. Reference Owen, Martinez and Powles2014; Schwartz-Lazaro et al. Reference Schwartz-Lazaro, Norsworthy, Scott and Barber2017). It is commonly attributed to two primary mechanisms. In the first, mutations occurring within the target enzyme represent a mechanism of resistance to herbicides with the same site of action (Délye Reference Délye2005; Yu et al. Reference Yu, Han and Powles2008). The second multiple herbicide resistance mechanism is conferred through non–target site resistance (NTSR) mechanisms, which can confer unprecedented resistance to multiple herbicide sites of action, including herbicides not yet discovered (Ahmad-Hamdani et al. Reference Ahmad-Hamdani, Yu, Han, Cawthray, Wang and Powles2013; Délye Reference Délye2013).
Rigid ryegrass (Lolium rigidum Gaudin) is a genetically diverse, obligate-outcrossing weed species present across the southern Australian cropping system and has evolved resistance to multiple herbicide sites of action (Boutsalis et al. Reference Boutsalis, Gill and Preston2012; Owen et al. Reference Owen, Walsh, Llewellyn and Powles2007). During, the 1980s and 1990s, in-season management of L. rigidum was effectively achieved with the selective POST herbicides diclofop-methyl (Group 1(A): inhibitors of acetyl CoA carboxylase [ACCase]) and chlorsulfuron (Group 2(B): inhibitors of acetolactate synthase [ALS]). However, resistance evolved rapidly, and Heap and Knight (Reference Heap and Knight1986) first reported the evolution of field-selected cross-resistance. Reports indicate resistance to ACCase- and ALS-inhibiting herbicides is widespread across southern Australia (Boutsalis et al. Reference Boutsalis, Gill and Preston2012; Malone et al. Reference Malone, Boutsalis, Baker and Preston2014; Yu et al. Reference Yu, Han and Powles2008). Increased reliance on the dinitroaniline herbicide trifluralin (Group 3(K1): inhibitors of microtubule assembly) came in response to widespread ACCase- and ALS-inhibitor resistance. Evolution of resistance to trifluralin has been widely documented across southern Australia (Broster and Pratley Reference Broster and Pratley2006). The release of the PRE herbicides prosulfocarb (Group 8(N): inhibitor of fat synthesis) and pyroxasulfone (Group 15(K3): inhibitors of very-long-chain fatty-acid synthesis) has provided effective options for controlling multiple-resistant L. rigidum in cereals (Boutsalis et al. Reference Boutsalis, Gill and Preston2014). Resistance evolution to the thiocarbamates, chloroacetamides, and pyroxasulfone would significantly diminish herbicide options available to growers for managing L. rigidum in cereals (Walsh et al. Reference Walsh, Fowler, Crowe, Ambe and Powles2011).
Resistance evolution to thiocarbamates and pyroxasulfone has been documented in only a few weed species, including L. rigidum. Busi et al. (Reference Busi, Gaines, Walsh and Powles2012) first reported metabolic pyroxasulfone resistance evolution in a low-dose recurrently selected population that had confirmed metabolic resistance to multiple site of action herbicides. Furthermore, unexpected cross-resistance evolution to prosulfocarb and S-metolachlor was shown in the population MR P6, greenhouse-grown progeny of a biotype selected through recurrent low doses of the herbicide pyroxasulfone (Busi and Powles Reference Busi and Powles2016). Resistance to triallate has been documented in wild oat (Avena fatua L.) in Canada (Kern et al. Reference Kern, Colliver, Maxwell, Fay and Dyer1996a). However, more recently, Mangin et al. (Reference Mangin, Hall and Beckie2016) documented a population that exhibited resistance to triallate, but also cross-resistance to the herbicides pyroxasulfone and sulfentrazone. Pyroxasulfone is a relatively new herbicide in Australia (Boutsalis et al. Reference Boutsalis, Gill and Preston2014), yet recently Brunton et al. (Reference Brunton, Boutsalis, Gill and Preston2018) reported the first case of field-evolved cross-resistance to prosulfocarb, triallate, and pyroxasulfone in a population of L. rigidum in South Australia.
The evolution of resistance to thiocarbamates and chloroacetamides, and more recently pyroxasulfone, highlights the significant threat that NTSR places on the long-term sustainability of new site of action herbicides (Busi and Powles Reference Busi and Powles2016). The extent of resistance to chloroacetamides and pyroxasulfone in L. rigidum populations is not yet fully understood. The objective of this study was to determine the level of cross-resistance to thiocarbamates, chloroacetamides, and pyroxasulfone in six field-evolved L. rigidum populations from the major cropping regions in southern Australia.
Materials and methods
Plant material
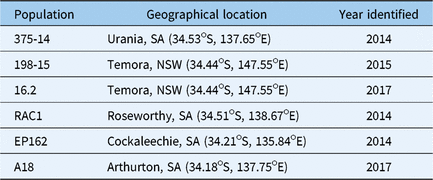
The seeds of L. rigidum populations 375-14 (R), 198-15 (R), 16.2 (R), and A18 (R) used in this study were collected from cropping fields across southern Australia (Table 1). These populations were collected from areas with a long history of crop production and use of herbicides. Population RAC1 (R) represents survivors from 1 million SLR4 seeds exposed to 6,000 g ha−1 triallate in the field in 2014. Surviving individuals were collected and seed bulked. Preliminary testing of field populations revealed resistance to multiple PRE herbicide sites of action, including microtubule assembly and fat synthesis. Two well-characterized herbicide-susceptible L. rigidum populations, SLR4 and VLR1 (S), and one confirmed herbicide-resistant population, EP162, were also used in this study (Boutsalis et al. Reference Boutsalis, Gill and Preston2012; Brunton et al. Reference Brunton, Boutsalis, Gill and Preston2018).
Collection sites for L. rigidum populations and their year of identification

Seedling growth and herbicide application
Seed from SLR4, VLR1, 375-14, 198-15, 16.2, EP162, A18, and RAC1 were weighed (0.2 g = 50 to 60 seeds) and spread onto the surface of 9.5 cm by 8.5 cm by 9.5 cm punnet pots (Masrac Plastics, Dry Creek, SA, Australia) containing cocoa peat potting mix, as described by Boutsalis et al. (Reference Boutsalis, Gill and Preston2012). Herbicides were applied immediately using a laboratory spray cabinet equipped with flat-fan nozzles (Hardi ISO F-110-01, Hardi, Adelaide, SA, Australia) delivering 118 L ha−1 of water at a pressure of 4 kPa. Control pots were not treated with any herbicide. The experiment was conducted and repeated outdoors under natural growing conditions in winter during the normal growing season (May to July 2018). Pots were watered as needed to maintain potting mix near field capacity. There were three replicates for each herbicide dose, and pots were arranged in a randomized complete block design.
Dose–response experiment
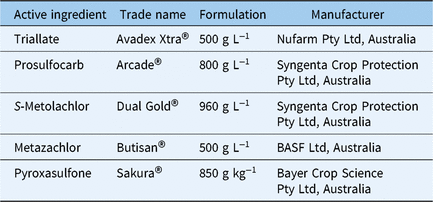
The five PRE herbicides were applied (Table 2) following the method described by Boutsalis et al. (Reference Boutsalis, Gill and Preston2012). The PRE herbicide prosulfocarb was applied to susceptible (S) biotypes at 75, 150, 300, 600, 1,200, and 2,400 g ha−1 and to resistant (R) biotypes at 600, 1,200, 2,400, 4,800, 9,600, and 19,200 g ha−1; the recommended label rate for L. rigidum control is 2,400 g ha−1. Triallate was applied to S biotypes at 50, 100, 200, 400, 800, and 1,600 g ha−1 and to R biotypes at 400, 800, 1,600, 3,200, 6,400, and 12,800 g ha−1; in Australia the recommended label rate of triallate for L. rigidum control is 1,500 g ha−1. S-Metolachlor was applied to S biotypes at 15, 30, 60, 120, 240, and 480 g ha−1 and to R biotypes at 120, 240, 480, 960, 1,920 and 3,840 g ha−1; the recommended label rate for L. rigidum control in Australia is 480 g ha−1. Metazachlor was applied to S biotypes at 28.12, 56.25, 112.5, 225, 450, and 900 g ha−1 and to R biotypes at 225, 450, 900, 1,800, 3,600, and 7,200 g ha−1; the recommended label rate for L. rigidum control is 900 g ha−1. Pyroxasulfone was applied to S biotypes at 3.2, 6.4, 12.8, 25.5, 51, and 102 g ha−1 and to R biotypes at 25.5, 51, 102, 204, and 408 g ha−1; the recommended label rate for L. rigidum control is 100 g ha−1. Pots were assessed 28 d after herbicide treatment, and plants that had emerged and grown to the 2-leaf stage were counted. Percentage survival was assessed as the number of plants growing in the treated pots compared with the average number present in the control pots.
Active ingredients, formulations, and manufacturers of herbicides used in dose–response experiments

Statistical analysis
Following ANOVA, data from both experimental runs were pooled, as there was no statistical difference between the experimental runs. The data were analyzed using a log-logistic equation (GraphPad Prism v. 7.0, GraphPad Software, San Diego, CA) fit to the percentage emergence data (Sakuma Reference Sakuma1998). To estimate no difference between estimated LD50 (dose required to reduce survival by 50% of individuals in the population) values, a t-test was conducted under the null hypothesis of R versus S populations showing no difference or having a ratio equal to 1 (Ritz et al. Reference Ritz, Baty, Streibig and Gerhard2015). LD50 parameter estimates from the log-logistic analysis were used to calculate the resistance index (RI), which is the R/S ratio of the LD50. The model fit was
 $$y\,\,{\rm{ = }}\,{{{\rm{100}}} \over {{\rm{1 + 10}}{{\rm{}}^{{\rm{(logI}}{{\rm{C}}_{{\rm{50}}}}{\rm{-}}x{\rm{) \times }}b}}}}$$
where y represents plant survival (%) or biomass reduction (%), x is the log-dose of the herbicide used, IC50 is the herbicide dose required to cause 50% reduction in plant emergence (LD50), and b denotes the slope of the curve.
Results and discussion
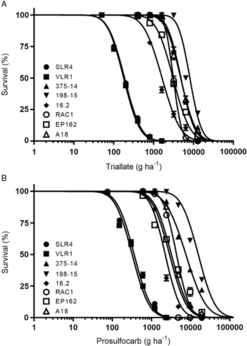
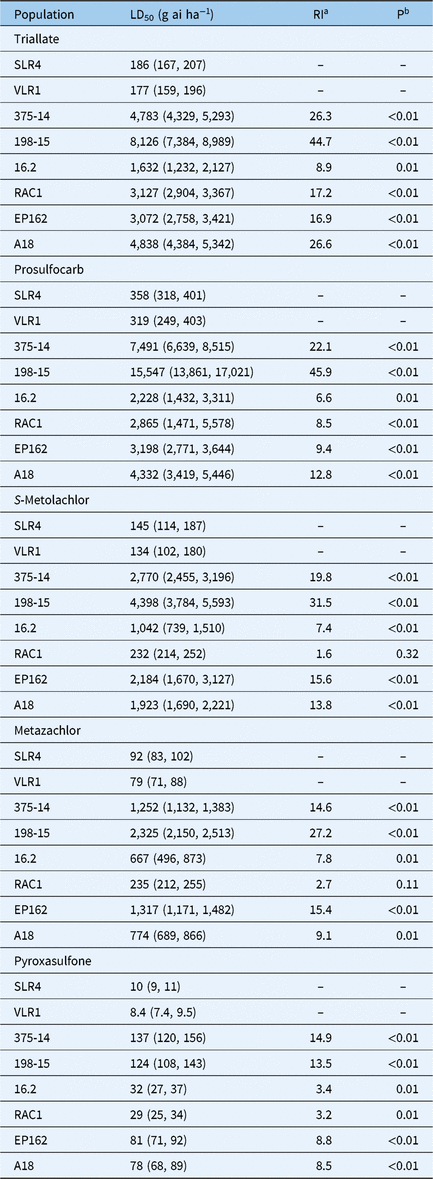
The SLR4 and VLR1 populations were completely controlled by triallate at the recommended field rate of 1,500 g ha−1. Resistant populations 375-14, 198-15, RAC1, EP162, and A18 showed no mortality, while population 16.2 showed 40% survival at this rate (Figure 1A). The triallate rates required for 50% mortality (LD50) for populations SLR4 and VLR1 were 186 and 177 g ha−1, respectively, and ranged from 1,632 to 8,126 g ha−1 for the R populations. The RI for triallate was 8.9- to 44.7-fold greater than the mean of both S populations (Table 3).
Response of SLR4, VLR1, 375-14, 198-15, 16.2, RAC1, EP162, and A18 populations of Lolium rigidum treated with varying rates of triallate (A) and prosulfocarb (B). Each data point is the mean of six replicates, and bars represent the standard error of the mean.

Pooled dose–response data for triallate, prosulfocarb, S-metolachlor, metazachlor, and pyroxasulfone required for 50% mortality (LD50) of resistant and susceptible Lolium rigidum populations with 95% confidence intervals (in parentheses) and resistance index (RI)

a RI as compared with the averages of standard susceptible populations (SLR4 and VLR1).
b Probability value (P) indicates significant difference in LD50 values between L. rigidum populations treated with a particular herbicide.
Prosulfocarb completely controlled the SLR4 and VLR1 populations at the recommended field rate of 2,400 g ha−1. In contrast, populations 375-14 and 198-15 showed complete survival at this rate (Figure 1B). All L. rigidum populations treated with prosulfocarb showed lower plant survival than with triallate at the recommended rate, with A18, RAC1, EP162, and 16.2 recording 88%, 81%, 72%, and 30% survival, respectively, at the recommended rate of prosulfocarb. The LD50 values for SLR4 and VLR1 were 358 and 319 g ha−1, respectively, and ranged from 2,228 to 15,547 g ha-1 for the R populations. Populations 375-14 and 198-15 showed similar RI values when treated with triallate and prosulfocarb compared with RAC1, EP162, and A18, which showed much lower RI values for prosulfocarb compared with triallate.
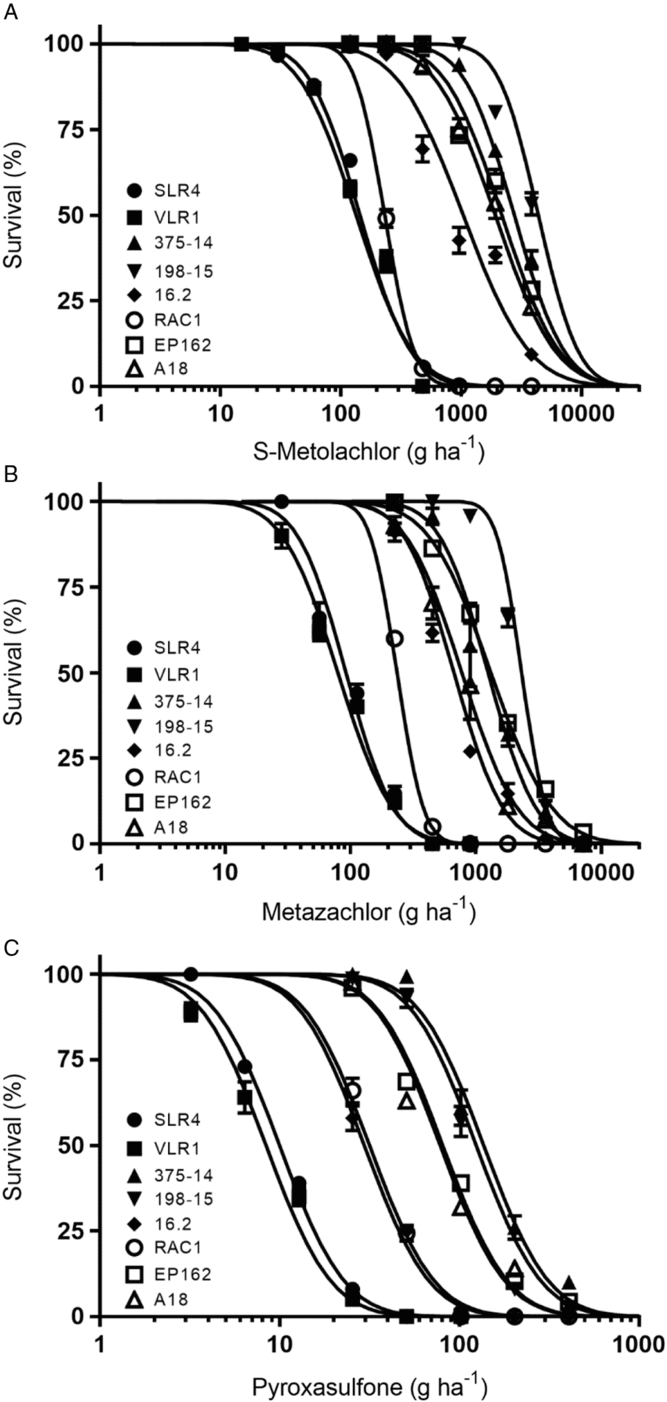
The SLR4, VLR1, and RAC1 populations were completely controlled by S-metolachlor at the recommended field rate of 480 g ha−1. The R populations A18 and 16.2 showed 95% and 62% survival at 480 g ha−1, respectively, while 375-14, 198-15, and EP162 showed no mortality at this rate (Figure 2A). The R populations 375-14, 198-15, 16.2, EP162, and A18 recorded RIs that were 19.8-, 31.5-, 7.4-, 15.6-, and 13.8-fold greater, respectively, than the S populations (Table 3).
Response of SLR4, VLR1, 375-14, 198-15, 16.2, RAC1, EP162, and A18 populations of Lolium rigidum treated with varying rates of S-metolachlor (A), metazachlor (B), and pyroxasulfone (C). Each data point is the mean of six replicates and bars represent the standard error of the mean.

Metazachlor completely controlled both S populations and the R population RAC1 at the recommended field rate of 900 g ha−1. All other populations were not completely controlled by metazachlor (Figure 2B), with the R populations 198-15, EP162, 375-14, A18, and 16.2 showing 95%, 66%, 38%, 55%, and 47% survival at the recommended rate, respectively. The LD50 values for SLR4, VLR1, and RAC1 were 92, 79, and 235 g ha−1 metazachlor, respectively (Table 3). Resistant populations 375-14, 198-15, 16.2, EP162, and A18 were 14.6-, 27.2-, 7.8-, 15.4-, and 9.1-fold more resistant to metazachlor, respectively, than SLR4 and VLR1.
Pyroxasulfone completely controlled SLR4, VLR1, and RAC1 at the recommended rate of 100 g ha−1. The LD50 values for the SLR4, VLR1, and RAC1 populations were 10, 8.4, and 29 g ha−1, respectively (Table 3). Populations 375-14, 198-15, A18, EP162, and 16.2 showed 61%, 57%, 39%, 32%, and 4% survival, respectively, at the recommend rate of pyroxasulfone (Figure 2C). The RI of the R populations ranged from 3.2- to 14.9-fold compared with the S populations. Except for populations 375-14 and RAC1, all R populations had lower levels of resistance to pyroxasulfone than to S-metolachlor or metazachlor.
Populations 375-14, 198-15, 16.2, RAC1, EP162, and A18 all demonstrated resistance to the thiocarbamate herbicides. Populations 375-14, 198-15, 16.2, EP162, and A18 displayed resistance to pyroxasulfone and in addition resistance to metazachlor and S-metolachlor. In a previous study, Brunton et al. (Reference Brunton, Boutsalis, Gill and Preston2018) reported resistance to the thiocarbamate herbicides and pyroxasulfone in EP162. A level of cross-resistance to chloroacetamides was previously reported by Burnet et al. (Reference Burnet, Barr and Powles1994) in L. rigidum populations with a long and complex history of exposure to herbicides. In this study, we show a higher level of cross-resistance between thiocarbamates, chloroacetamides, and pyroxasulfone in field-selected populations 375-14, 198-16, 16.2, EP162, and A18 that will likely result in field failures with thiocarbamate herbicides. Furthermore, L. rigidum populations with resistance to triallate also showed resistance to prosulfocarb (Table 3). The RI to these two herbicides varied slightly for several of the populations, with greater resistance to triallate than prosulfocarb, which is consistent with the findings reported by Brunton et al. (Reference Brunton, Boutsalis, Gill and Preston2018).
The level of resistance to thiocarbamate herbicides observed in this study was much greater than previously reported in other weed species (Beckie et al. Reference Beckie, Warwick and Sauder2012; Kern et al. Reference Kern, Colliver, Maxwell, Fay and Dyer1996a; Keshtkar et al. Reference Keshtkar, Mathiassen, Moss and Kudsk2015). Thiocarbamate herbicides require conversion into a toxic metabolite within plants to exert their herbicidal effects. The activation of thiocarbamate herbicides in plants involves the oxidation of the parent compound into the toxic sulfoxide via cytochrome P450 enzymes (Casida et al. Reference Casida, Gray and Tilles1974; Fuerst Reference Fuerst1987). The sulfoxide is subsequently conjugated through the involvement of glutathione S-transferase and cleaved into the cysteine conjugate (Hubbell and Casida Reference Hubbell and Casida1977; Shimabukuro Reference Shimabukuro1975). According to Kern et al. (Reference Kern, Peterson, Miller, Colliver and Dyer1996b), the primary mechanism for triallate resistance in A. fatua was reduced herbicide activation. This is consistent with the results for the populations 375-14, 198-15, 16.2, RAC1, EP162, and A18 treated with triallate and prosulfocarb and could suggest a similar resistance mechanism conferring resistance to these herbicides.
The involvement of glutathione S-transferases (GSTs) has previously been shown to confer crop selectivity to several different chloroacetamide herbicides (Fuerst Reference Fuerst1987; Lamoureux et al. Reference Lamoureux, Shimabukuro, Frear, Caseley, Cussans and Atkin1991). he same mechanism may also confer resistance to chloroacetamides and pyroxasulfone in the L. rigidum populations 375-14, 198-15, EP162, A18, and 16.2. The resistance mechanism would likely be similar to that conferring tolerance to pyroxasulfone, as described by Tanetani et al. (Reference Tanetani, Ikeda, Kaku, Shimizu and Matsumoto2013) in wheat (Triticum aestivum L.) and Busi et al. (Reference Busi, Porri, Gaines and Powles2018) in a pyroxasulfone-resistant population of L. rigidum. Similarly, Mangin et al. (Reference Mangin, Hall and Beckie2016) showed cross-resistance to pyroxasulfone and sulfentrazone in a triallate-resistant A. fatua population in Canada and suggested enhanced metabolism by P450s. We suggest the possibility of multiple resistance mechanisms involving P450s and increased GST activity, similar to those reported in wheat, conferring resistance in the L. rigidum populations 375-14, 198-15, 16.2, EP162, and A18. A single resistance mechanism, most likely loss of specific P450s in the triallate-selected population RAC1, could explain the observed resistance to thiocarbamates but susceptibility to chloroacetamides and pyroxasulfone, due to the herbicide not being activated (Kern et al. Reference Kern, Peterson, Miller, Colliver and Dyer1996b).
Evolution of cross-resistance to herbicides can occur through an assortment of resistance-endowing traits (Délye et al. Reference Délye, Jasieniuk and Le Corre2013) selected through repeated application of the same herbicide (Beckie and Tardif Reference Beckie and Tardif2012). The current understanding of NTSR remains limited (Yu and Powles Reference Yu and Powles2014), which makes the evolution of cross-resistance to other site of action herbicides difficult to predict. Resistance to the herbicide pyroxasulfone has been shown to be conferred by single semidominant genetic traits that resulted in the rapid evolution of cross-resistance to thiocarbamate herbicides (Busi et al. Reference Busi, Gaines, Vila-Aiub and Powles2014). Plant survival in L. rigidum populations 375-14 (61%) and 198-15 (57%) treated with the label recommended rate of pyroxasulfone is consistent with the level of survival observed by Busi and Powles (Reference Busi and Powles2016) in their 6th cycle of low-dose recurrent selection in this species. In contrast, RAC1, which was selected with a single application of 6,000 g ha−1 triallate, only showed resistance to thiocarbamate herbicides. This population was successfully controlled with the field rates of S-metolachlor, metazachlor, and pyroxasulfone.
This study has demonstrated multiple L. rigidum populations in southern Australia with varying extents of resistance to the herbicides triallate, prosulfocarb, S-metolachlor, metazachlor, and pyroxasulfone. The evolution of cross-resistance between these sites of action in L. rigidum threatens the viability of weed control in cereals in Australia. Currently, there are no remaining herbicides that are able to control these herbicide-resistant L. rigidum populations in cereals. Evolution of resistance to trifluralin has been successfully managed so far with the use of prosulfocarb and pyroxasulfone and integration of nonchemical weed control tactics in cereal crops. Late-season crop-topping has been shown to be an effective strategy for reducing the amount of viable seed being returned to the weed seedbank (Kleemann et al. Reference Kleemann, Preston and Gill2016). In addition to selective herbicides, a diverse array of cultural and nonherbicidal weed control tactics should be implemented to manage L. rigidum populations (Beckie Reference Beckie2006; Walsh and Powles Reference Walsh and Powles2007). These would help minimize resistance evolution and allow sustained long-term herbicide use. There is a risk that resistance evolution to thiocarbamates, chloroacetamides, and pyroxasulfone would result in increased reliance on the few remaining effective herbicides, such as propyzamide, and this may accelerate evolution of resistance to those herbicides.
Author ORCID
David J. Brunton https://orcid.org/0000-0001-9694-904X
Acknowledgments
The authors acknowledge the Grains Research and Development Corporation for funding this research. No conflicts of interest have been declared.