Introduction
Cabbage is an important agricultural crop that occupies a central role in the economy of many countries, especially in Asia and Africa (Grzywacz et al., Reference Grzywacz, Rossbach, Rauf, Russell, Srinivasan and Shelton2010). The diamondback moth (DBM) Plutella xylostella (L.) (Lepidoptera: Plutellidae) is an oligophagous pest, considered as the most important source of crop losses in the Brassicaceae family (van Loon et al., Reference van Loon, Wang, Nielsen, Gols and Qiu2002; Shelton, 2004; Sarfraz et al., Reference Sarfraz, Dosdall and Keddie2006). Annual costs for pest management expenses are estimated at US$ 1 billion (Grzywacz et al., Reference Grzywacz, Rossbach, Rauf, Russell, Srinivasan and Shelton2010) exclusively for synthetic insecticide applications. Complete dependence on a chemical-based strategy for crop protection is, however, not sustainable. Also, the DBM has developed resistance to many synthetic insecticides and biopesticides, including Bacillus thuringiensis (Berliner) formulations (Liu et al., 1997; Zhou et al., Reference Zhou, Huang and Xu2011). As a result, attention has been directed towards alternative methods that could be used as components of integrated pest management systems.
Biological control using parasitoids (Lim, 1992) is an alternative to chemical control. Among other natural enemies of DBM, the larval parasitoid Oomyzus sokolowskii Kurdjumov (Hymenoptera: Eulophidae) is one of the most important endoparasitoids, used as a biological control agent for DBM management in various parts of the world (Wang et al., Reference Wang, Liu, Gao and Lin1999; Ferreira et al., Reference Ferreira, Barros and Torres2003).
Efficient biological control is only possible through knowledge of the biology and ecology of both the pest and its natural enemies (Andow et al., 1997; Martinez-Castillo et al., Reference Martinez-Castillo, Leyva, Cibrian-Tovar and Bujanos-Muñoz2002). DBM populations from different localities present differences in biological behaviour (Arvanitakis et al., 2002; Kirk et al., 2004). Previous studies have demonstrated the existence of genetic variations between various DBM populations (Pichon et al., 2004; Roux et al., Reference Roux, Gevrey, Arvanitakis, Gers, Bordat and Legal2007). A parasitoid host can affect its performance, especially in gregarious species (Silva-Torres et al., Reference Silva-Torres, Filho, Torres and Barros2009b). To date, little is known about the performance of O. sokolowskii, taking into account those biotic factors. The knowledge of such differences could be used in biological control or in conservation biological control programmes against the DBM.
Hence, the aim of this study was to describe the interactions between P. xylostella larvae and O. sokolowskii females under laboratory conditions. We focused on the effect of gregarious behaviour, host origin and stages, and female parasitoid age on the parasitism rate, developmental time, the number of offspring and the sex ratio of O. sokolowskii.
Materials and methods
Study site
The experiments were conducted at the Laboratory of Entomology for International Cooperation in Agronomic Research for Development Centre (CIRAD) in Montpellier, France.
Insect rearing
DBM larvae were previously collected from cabbage plantations (Brassica oleracea var. capitata L.) in the Niayes area in Senegal (12°54′44″N and 12°8′84″NW; 189 m elevation). The colony was maintained on Chinese mustard (Brassica juncea (L.) Czern.), where gravid females were allowed to oviposit. Emerging larvae were placed on the fresh leaves of cauliflower (B. oleracea var. botrytis L.) for their development. The larvae were later transferred onto the fresh leaves placed on the bottom of a large transparent plastic box (28 × 26 × 15 cm), for pupation, and pupae were collected daily. Newly emerged adults were placed in cages (50 × 50 × 50 cm) and fed with water and honey.
The O. sokolowskii colony was obtained from parasitized DBM pupae collected from cabbage plantations in Pikine (near Dakar), Senegal. The rearing consisted of exposing fourth-instar DBM larvae to parasitoid females in transparent plastic boxes (8 × 5 cm) for oviposition for 24 h. The DBM larvae were removed after parasitism and placed in identical boxes for their development until pupation. Fresh leaves of cauliflower were provided as source of food. Adult parasitoids emerging from parasitized pupae were collected and maintained in a plastic box and fed with honey drops deposited on the mesh cover.
Climatic conditions of all insect rearing were maintained at 25 ± 1°C temperature, 60 ± 5% relative humidity and 12 h light-12 h dark photoperiod.
Gregariousness of O. sokolowskii
Females of O. sokolowskii (24 h old) were used in this experiment. In brief, 1, 5, 10, 15 and 20 females were placed, respectively, with 2, 10, 20, 30 and 40 fourth-instar DBM larvae (from Senegal) for 24 h. The number of host larvae was increased to avoid the risk of superparasitism. The larvae were then transferred individually into clear plastic pill boxes (3.5 × 1 cm) with a leaf disc of cabbage as food supply, and monitored daily until the emergence of adult parasitoids. The parasitism rate was calculated from the number of parasitized larvae and pupae. The developmental time (from egg to adult), and the number of offspring and the sex ratio were also compared in each cohort. The experiment was replicated seven times.
Host origin effects
Two populations of P. xylostella were used in this experiment: a population from Senegal (from the Niayes area) and another one from Martinique Island (Saint Pierre, 14°44′30″N and 61°10′33″W; 1200 m elevation). For each population, the size of the pupae was measured using a dissecting microscope equipped with an ocular micrometer. Thirty pupae were used for each DBM population.
Fifteen 24-h-old O. sokolowskii females were exposed to 30 fourth-instar DBM larvae from each of the regions. After 24 h of exposure, all larvae were collected and placed individually in clear plastic pill boxes and followed up until the emergence of adult parasitoids. The parasitism rate was calculated from the number of parasitized larvae and pupae of each population. The developmental time (from egg to adult), and the number and sex ratio (% females) of the offspring were calculated. Bioassays were replicated seven times.
DBM stage effects
Thirty DBM larvae (second, third and fourth), pre-pupae and pupae were exposed to 15 O. sokolowskii females in a clear plastic pill box for 24 h. The DBM population in this experiment was native to Senegal. Honey drips were deposited on the cover mesh as food supply. Parasitized larvae were transferred separately into pill boxes, with a leaf disc of cabbage as food supply. The newly formed pupae were monitored until the emergence of parasitoid adults. The parasitism rate for each DBM stage was calculated from the number of parasitized pupae. The developmental time (from egg to adult), the number of offspring and the sex ratio (% female) of parasitoids were compared among the different host stages. The experiment was replicated 10 times for each DBM stage.
Effect of female parasitoid age
Fifteen 1-, 5-, 15- and 28-day-old O. sokolowskii females were, respectively, exposed to 30 fourth-instar DBM larvae for 24 h. The larvae were collected and transferred individually into pill boxes. They were monitored until the emergence of parasitoids. The parasitism rate, developmental time, the number of offspring and the sex ratio (% females) were compared. For each cohort, the experiment was replicated five times.
Statistical analysis
Data were normalized by logarithmic transformation before being subjected to an analysis of variance (ANOVA). Parasitism rate, the total number of adult offspring, developmental time and offspring sex ratios were compared for the different treatments using one-way ANOVA. Means were separated using the Student–Newman–Keuls test (XLSTAT software, version 2012.1.01). Parasitism rate, developmental time, parasitoid offspring number and sex ratio between host populations of different origins were compared with t-tests (STATVIEW, 1996). The sex ratio was calculated using the Silva-Torres et al. (Reference Silva-Torres, Filho, Torres and Barros2009b) formula as the proportion of females. In all statistical analyses, the level of significance was kept at 5%.
Results
Gregariousness of O. sokolowskii
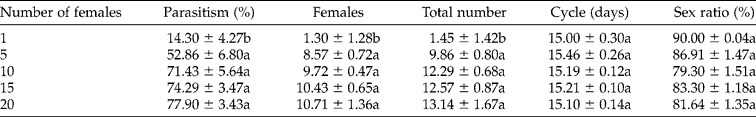
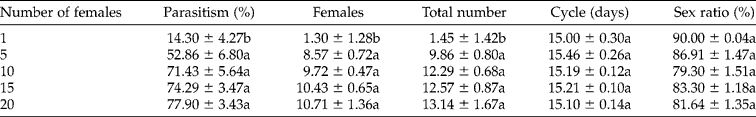
The parasitism rate varied significantly according to the number of females (F (4,24)= 11.35; P< 0.0001; Table 1). The parasitism rate was significantly lower at one female parasitoid and increased as the number of females increased. However, there were no significant differences between the 5, 10, 15 and 20 females (P< 0.05). There were significant differences between the number of female parasitoids on the number of adults (F (4,24)= 17.80; P< 0.0001), and the number of females (F (4,24)= 16.50; P< 0.0001). A single female produced fewer offspring than grouped females. The developmental time and the sex ratio of the progeny were not significantly affected by the number of female parasitoids (F (4,24)= 1.32; P= 0.29 and F (4,24)= 3.94; P= 0.05, respectively; Table 1).
Mean (±SE) parasitism rate, productivity, developmental time and sex ratio (% female) of Oomyzus sokolowskii on DBM larvae
Means in columns followed by the same letters are not significantly different (P>0.05; Student–Newman–Keuls test).
Host origin effects
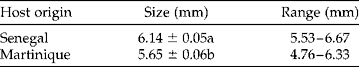
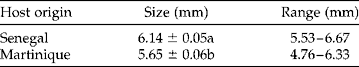
The difference in size between DBM pupae from Senegal and DBM pupae from Martinique was significant (t= 6.091; degree of freedom (df) = 58; P< 0.0001). DBM populations from Senegal were morphologically bigger than those from Martinique (Table 2).
Mean size of DBM pupae (mean±SE) from different geographic origins
Means in columns followed by the same letter are not significantly different (P>0.05; t-test).
There was a significant difference in parasitism rate between DBM populations from Senegal and Martinique (t= − 2.62; df = 12; P= 0.022; Table 3). However, there was no significant difference in the total production of adults and the production of females (t= − 1.31; df = 12; P= 0.215 and t= − 0.52; df = 12; P= 0.61, respectively). The number of males in the offspring was significantly different between the two populations (t= − 2.68; df = 12; P= 0.02). There was no significant difference in developmental time between the two populations (t= 0.60; df = 12; P= 0.56). The sex ratio was significantly different between the two populations (t= 2.52; df = 12; P= 0.026; Table 3).
Effect of host origin on the parasitism rate, progeny, developmental time and sex ratio (mean±SE) of Oomyzus sokolowskii

Means in columns followed by the same letters are not significantly different (P>0.05; t-test).
DBM stage effects
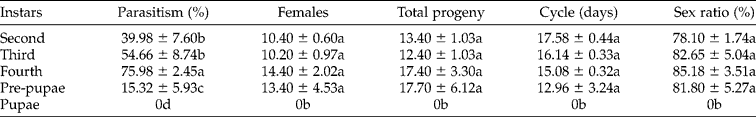
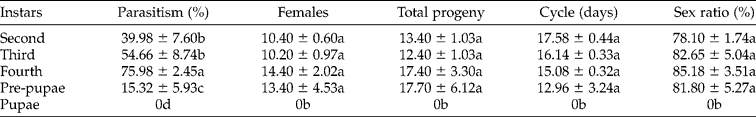
The parasitism rate varied significantly according to host stage (F (4,36)= 26.23; P< 0.0001). It was higher in L4 larvae and lower in pre-pupae by 75.9 and 15.3%, respectively. However, there were no significant differences between the L2 and L3 larval stages (Table 4). Similarly, there were no significant differences in the total production of adults (F (3,27)= 0.50; P= 0.68) and females (F (3,27)= 0.69; P= 0.57) between the host stages. Developmental time and sex ratio were not different between the host stages (F (3,27)= 1.39; P= 0.28 and F (3,27)= 0.56; P= 0.65, respectively; Table 4).
Effect of host stages on the parasitism rate, progeny, developmental time and sex ratio of the DBM parasitoid Oomyzus sokolowskii
Means in columns followed by the same letters are not significantly different (P>0.05; Student–Newman–Keuls test).
Effect of female parasitoid age
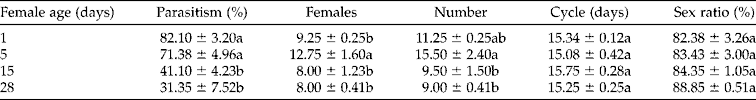
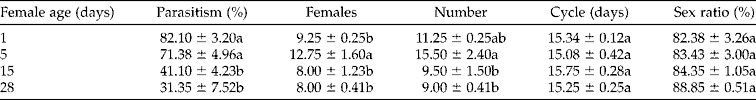
The parasitism rate was significantly affected by the age of O. sokolowskii females (F (3,12)= 21.32; P< 0.0001; Table 5). It was higher in 1- and 5-day-old females. The number of females was significantly affected by the age of female parasitoids (F (3,12)= 4.70; P= 0.02); it was higher in 5-day-old female parasitoids. The number of adults was also significantly affected (F (3,12)= 4.24; P= 0.03). However, the developmental time and the sex ratio were not affected by the age of female parasitoids (F (3,12)= 1.01; P= 0.42 and F (3,12)= 1.55; P= 0.25, respectively).
Effect of female Oomyzus sokolowskii age on parasitism rate, the number of offspring, developmental time and sex ratio (mean±SE)
Means in columns followed by the same letters are not significantly different (P>0.05; Student–Newman–Keuls test).
Discussion
Knowledge on the biology and ecology of biological control agents is of paramount importance in the management of pests such as DBM. Our results suggest that gregariousness promotes increased parasitism rates and increased number of offspring per female. In fact, gregariousness is related to superparasitism, which, in turn, favours a higher number of offspring (Gu et al., Reference Gu, Wang and Dorn2003; Silva-Torres and Matthews, Reference Silva-Torres and Matthews2003; Keasar et al., Reference Keasar, Segoli, Bakar, Steinberg and Giron2006). According to Silva-Torres et al. (Reference Silva-Torres, Filho, Torres and Barros2009b), gregariousness and superparasitism can adversely affect parasitoid fitness. These behaviours appear to be of advantage to the parasitoid (Yamada and Miyamoto, Reference Yamada and Miyamoto1998). In our study, the parasitism rate and the number of offspring increased with the number of parasitoid females. These results corroborate those of Hirashima et al. (Reference Hirashima, Miura, Miura and Matsuda1990) who found that host availability was a favourable factor to high parasitism rates. The proportion of males in the offspring also increased with the number of female parasitoids. These results are similar to those reported by Chen et al. (Reference Chen, Zhang, Huangfu, Yao, Zhou and Kuhlmann2008).
The DBM population from Senegal seemed to be of higher fitness than the population from Martinique. According to Chown et al. (Reference Chown, Jumbam, Sorensen and Terblanche2009), large-sized insects have a higher chance of survival and reproduction. In our study, the parasitism rate was significantly higher in the population from Martinique; however, female productivity was similar in both populations. Our results do not seem to be in agreement with previous findings. Edwards (Reference Edwards1954) has reported the effect of host size. The author discovered that most female parasitoids, especially in gregarious species, first estimate the size of the host before ovipositing. This trait is one of the most important indicators used by female parasitoids for reproduction (Aruna and Manjunath, Reference Aruna and Manjunath2010). Zaviezo and Mills (Reference Zaviezo and Mills2000) made the same assertion; the offspring production in gregarious parasitoids is often correlated with host size. In our results, DBM pupae from Senegal are larger than the DBM from Martinique, which would imply that the female parasitoid would oviposit more in Senegalese larvae. Yet, DBM individuals from Senegal, which were bigger in size, were less parasitized ( − 15%). Although the number of females was similar, the number of males in the offspring was higher in DBM individuals from Martinique. As a result, the sex ratio was higher in Senegalese DBM, which implies that O. sokolowskii could be a more efficient biological control agent in Senegal than in Martinique. In addition to the difference in size between the DBM populations, the difference in altitude between the regions could explain the difference in the performance of O. sokolowskii (Shelly et al., Reference Shelly, Rendon, Hernandez, Salgado, McInnis, Villalobos and Liedo2003). It has been shown that distributions of both hosts and their parasitoids are influenced by altitude (Sivinski et al., Reference Sivinski, Jeronimo and Holler2000, Reference Sivinski, Aluja, Piñero and Qjeda2004), which presumably is, in turn, due to temperature and moisture gradients.
The study revealed the importance of host stage as an important ecological parameter to be considered in the biology of parasitoids (Bai et al., Reference Bai, Luck, Forster, Stephens and Janssen1992; Godfray, Reference Godfray1994; Islam and Copland, Reference Islam and Copland1997; Fidgen et al., Reference Fidgen, Eveleigh and Quiring2000). It has also been shown that the quality of the host affects the fitness of offspring in parasitoids (Godfray, Reference Godfray1994). Our results indicate that the parasitism rate was higher in the fourth larval stages of DBM, which seems to be the most suitable stage for the development of O. sokolowskii. Host stages of bigger size contain more resources for the parasitoid larval stages (Harvey et al., Reference Harvey, Bezemer, Elzinga and Strand2004). These observations are similar to previous work reported by Talekar and Hu (Reference Talekar and Hu1996).
There were no significant differences in the number of offspring, developmental time and progeny sex ratio of O. sokolowskii in relation to the age of host stages, corroborating findings of Wang et al. (Reference Wang, Liu, Gao and Lin1999), possibly due to the gregariousness and superparasitism behaviour of O. sokolowskii. Although there were differences in parasitism rate between the stages of DBM, potential competition for resources between larval parasitoids could affect the number of offspring. Gregariousness and superparasitism can adversely affect the number of offspring (Silva-Torres et al., Reference Silva-Torres, Filho, Torres and Barros2009b). Consequences of such behaviour could greatly affect the fitness of progeny. On the other hand, Nakamura and Noda (Reference Nakamura and Noda2002) reported that the number of O. sokolowskii tends to increase with host age and is significantly higher in the late fourth-stadium hosts. Yet, our results did not corroborate their findings.
The success of parasitism depends on the age of the female parasitoid (Medeiros et al., Reference Medeiros, Ramalho, Lemos and Zanuncio2000); generally, parasitism rate decreased with age as shown in our study that 5-day-old females lay more eggs in their host than older females. This decrease in productivity can be explained by a decrease in physiological activity (Giron and Casas, Reference Giron and Casas2003). Silva-Torres et al. (Reference Silva-Torres, Barros and Torres2009a) showed that the parasitism rate was higher in 2- to 4-day-old females of O. sokolowskii. According to Rajapakse (Reference Rajapakse1992), the ideal age for Cotesia marginiventris (Cresson) (Hymenoptera: Braconidae) to properly parasitize larvae of Spodoptera frugiperda (Smith) (Lepidoptera: Noctuidae) ranged from 48 to 96 h, whereas the ideal age of parasitism for Ceratogramma etiennei (Delvare) (Hymenoptera: Trichogrammatidae) varied from 1 to 2 days post-emergence (Amalin et al., Reference Amalin, Peña and Duncan2005). Our results are similar to the work of Silva-Torres et al. (Reference Silva-Torres, Barros and Torres2009a) and Chen et al. (Reference Chen, Zhang, Huangfu, Yao, Zhou and Kuhlmann2008), who showed that the progeny produced per female and the number of parasitoids emerging per host significantly decreased according to age. Similarly, Li et al. (Reference Li, Sirois, Lee, Maurice and Henderson1993) argued that offspring production from females of Trichogramma minutum Riley (Hymenoptera: Trichogrammatidae) decreases with age. However, the developmental time and sex ratio of offspring were not different between the different age groups of the parasitoid. Our results are similar to the findings of Riddick (Reference Riddick2003), who demonstrated that the age of Anaphes iole Girault (Hymenoptera: Mymaridae) does not affect the sex ratio of the parasitoid.
The parasitism rate tended to decrease drastically in the 5-days-old females, suggesting that beyond a certain period of maturity, O. sokolowskii females are less efficient in controlling DBM populations. Therefore, biological control of DBM cannot rely entirely on the use of parasitoids when they are too old (Persad and Hoy, Reference Persad and Hoy2003; Amalin et al., Reference Amalin, Peña and Duncan2005), and other methods need to be envisaged.
Conclusion
The present study confirms the importance of O. sokolowskii as a promising biological control agent that could be used in an augmentative approach for the management of DBM populations in cabbage production. However, performance could be affected by host geographical origin. Moreover, age of female parasitoids could be a limiting factor for parasitoid production; therefore, other parameters should be combined during DBM management. The results of this study show that it is necessary to know in real time the best period for parasitoid mass release to ensure successful parasitism of DBM populations.
Acknowledgements
This work was funded by the French Agency ‘Agence Universitaire de la Francophonie’ through the programme ‘Horizons Francophones’. We thank the French Agricultural Research for Development Centre (CIRAD) in Montpellier for providing all the research facilities. We thank Dr A. A. Kirk, researcher at the EBCL USDA-ARS in Montpellier, for English translation.